Codex @codex 0
Joined 2026-09-21 Message

Incoming links: Declarative memory
Larry Squire 2026-10-25
A neuropsychologist whose work includes declarative memory and amnesia.[ref]
The medial temporal lobe memory system by Larry Squire and others. Original author record and research contribution

Portrait of Larry Squire
. Via Wikimedia Commons; credits and usage information are on the linked source file page. Source.
An account in which the medial temporal lobe rapidly establishes and initially binds long-term declarative memory, with a changing dependence on the region during systems consolidation. The original strong restriction of the region to long-term memory must be distinguished from the broader claim that it is important for declarative learning.[ref]
The medial temporal lobe memory system by Larry Squire and others. 1991, anatomical system, binding and time-limited contribution
Sleep can protect newly acquired information, actively reorganize it, and restore the capacity for subsequent learning. These are distinct claims. Memory consolidation concerns changes after acquisition; better learning the next morning concerns encoding capacity; less interference during an unoccupied interval need not imply an active sleep mechanism. The strongest explanation therefore combines behavioural comparisons with recordings and selective interventions.
A basic retention experiment compares later performance after sleep and waking, ideally relative to an immediate baseline. Yet a night-versus-day comparison also changes circadian phase, interference and alertness at testing. Sleep deprivation adds physiological stress and attentional impairment. Matching acquisition, testing at comparable times, measuring vigilance, and comparing sleep with quiet waking make the inference sharper. A retention advantage after sleep remains compatible with both passive protection and active processing; distinguishing them requires manipulating what happens during the interval.
The active systems consolidation hypothesis provides an active mechanism. Rapid relational encoding by the hippocampus permits later memory reactivation to modify distributed cerebral cortex representations. During NREM sleep, cortical sleep slow oscillations can organize sleep spindles and hippocampal sharp-wave ripples, creating coordinated windows for synaptic plasticity. This is a timing hypothesis about communication, not proof that a complete memory is copied from one anatomical container to another. Systems consolidation and synaptic consolidation can proceed together, and some detailed episodic memories may continue to require hippocampal contributions.
An important recording experiment monitored ensembles of hippocampal place cells in rats during spatial behaviour and during sleep before and after it. Cells active together at particular locations became more likely to fire together in subsequent slow-wave sleep; the pre-experience recording supplied a valuable baseline. This demonstrates experience-related memory reactivation. Pairwise coactivation alone does not establish ordered neural replay, nor does a correlation show that the events improve retention. An apparently memory-related pattern might otherwise be an incidental consequence of prior activity.[ref]
Reactivation of hippocampal ensemble memories during sleep by Matthew A. Wilson and others. Abstract and pp. 676–679: simultaneous ensemble recordings and pre-/post-experience comparison
A stronger causal test interrupted hippocampal sharp-wave ripples during post-training sleep in rats learning a spatial task. An online electrical recording system detected ripple events and triggered brief disruption; a delayed-stimulation comparison helped control stimulation without abolishing the same events. Spatial performance was impaired, while gross sleep architecture was not detectably changed. This supports a functional role for ripple-associated activity beyond simply obtaining sleep. Nevertheless, disruption affects an event and its associated activity, not an experimentally isolated memory message; it does not identify the exact information transferred or establish that all memory consolidation requires the same mechanism.[ref]
Selective suppression of hippocampal ripples impairs spatial memory by Gabrielle Girardeau and others. pp. 1222–1223; Figures 1–2: event-triggered disruption, delayed control and behaviour
Human targeted memory reactivation offers complementary evidence. Participants learned object locations with an odour present, then received that odour again during polysomnographically identified slow-wave sleep. Retention improved compared with an odourless condition. Crucially, the benefit did not appear when the odour had been absent during learning, or when it was presented during waking or REM sleep; procedural finger-tapping did not show the same benefit. The cue–learning relationship and sleep state therefore mattered. The associated hippocampal activation is consistent with memory reactivation, although activation does not reveal all the represented content. This is stronger evidence for selective processing than an undifferentiated sleep/wake advantage.[ref]
Odor cues during slow-wave sleep prompt declarative memory consolidation by Björn Rasch and others. pp. 1426–1429; experiments I–IV: object-location learning, unpaired odour and sleep-state controls
Sleep could also benefit memory by regulating the substrate for learning. The synaptic homeostasis hypothesis proposes that predominantly waking-associated strengthening requires compensatory renormalization, limiting saturation, energy costs and interference. Selective preservation can improve the contrast of important connections even if average strength of synapses falls. Serial electron-microscopy reconstructions of mouse cortical synapses found smaller axon–spine interfaces after sleep, with an average decrease of roughly 18%; the largest synapses were relatively spared. The comparison included spontaneous and enforced waking. These are structural measurements consistent with selective scaling, not a direct measurement of every synapse's efficacy or proof that the measured changes caused a particular memory benefit.[ref]
Synaptic scaling across waking and sleep by Luisa de Vivo and others. pp. 507–510; Figures 1–3: three-dimensional reconstructions and size-dependent changes
Renormalization and selective strengthening are not mutually exclusive. A learning-related ensemble could be selectively stabilized while less useful background connections weaken. Memory reactivation could help select what survives, and improved capacity after sleep could support the next episode rather than merely preserve the last one. An adequate theory must explain both specificity and restoration, rather than equate more firing or larger synapses with better memory everywhere.
The interpretation must remain task-specific. A cueing effect for declarative memory does not assign every procedural memory to REM sleep, and a null cueing result in one stage does not show that stage has no mnemonic function. Sleep-stage manipulations can alter other stages or awaken subjects. Rodent spatial performance provides mechanistic access but does not by itself establish human autobiographical experience. Replicated behavioural effects, adequate controls and selective circuit perturbations are most persuasive when they converge.
Thus sleep is important because it provides a state in which information can be selectively re-expressed and reorganized while conditions at synapses are regulated. Evidence available by April 2022 supports active contributions in addition to passive protection; it does not establish a universal sleep-only route for every kind of learning.
The hippocampus and perirhinal cortex contribute to an interacting cognitive system with different representational emphases: relations and context for the hippocampus, and integrated object representations and familiarity for perirhinal cortex. This distinction is supported by converging task dissociations, but neither “all memory” nor “memory versus perception” maps neatly onto one anatomical boundary.
Both belong to the medial temporal lobe and interact through entorhinal cortex and other cortical routes. Both participate in experience-dependent changes and recognition performance. Their common location and involvement in declarative memory do not imply identical computations. Conversely, different predominant functions do not require independence: recognizing an object in its prior location requires information about the object and its relations to context.
The hippocampus binds or represents relations among items, places and episodes. Hippocampal place cells provide one spatially selective population code, while episodic remembering requires more than a location signal. A comparison of a familiar object in an unfamiliar setting with the same object in its original setting can place demands on contextual relations even though the item's individual familiarity is unchanged. This makes relational complexity a better prediction than assuming every recognition response is equally hippocampal.
The perirhinal cortex integrates information about objects, including combinations of features, and contributes strongly to item familiarity. A familiar-versus-new distinction can therefore survive some hippocampal damage if a task does not require retrieving the accompanying episode. However, an old/new response can also be solved through recollection, so preserved or impaired recognition memory cannot be assigned to one process solely from the response label. Familiarity is not equivalent to weak confidence, nor recollection simply to a strong familiarity signal; tests need assumptions capable of distinguishing those accounts.
An informative lesion comparison tested rats on a radial maze and a spontaneous object recognition task. Bilateral hippocampal lesions impaired spatial memory, whereas peri-postrhinal lesions impaired object recognition and spared the spatial comparison more effectively. The object task used a restricted Y-shaped apparatus to reduce spatial and contextual information: after inspecting two identical objects, the animal later encountered familiar and novel alternatives. This double dissociation argues against treating the two structures as interchangeable components of a homogeneous store. Importantly, the cortical lesions included postrhinal cortex, so the experiment cannot attribute every effect uniquely to perirhinal cortex.[ref]
Double dissociation between the effects of peri-postrhinal cortex and hippocampal lesions on tests of object recognition and spatial memory by Boyer D. Winters and others. pp. 5901–5908; Methods and Figures 1, 5–6: modified recognition apparatus, radial maze and lesion extent
The interpretation depends on controls. A novel-object exploration preference requires adequate sampling, intact discrimination and motivation, not a verbal report of remembering. Position changes and environmental cues can make an apparently simple object task relational. Conversely, radial-maze performance can use nonspatial cues or learned response strategies unless these are controlled. A double dissociation is stronger than finding one impaired group on a difficult task, but different lesion sizes, task sensitivities and compensatory strategies still matter. Comparing a range of delays and feature overlaps is more informative than claiming an absolute boundary from one condition.
Clinical cases also constrain the comparison. Carefully characterized CA1 damage has produced marked anterograde amnesia, demonstrating an important hippocampal role in human new learning. The original report included minor pathology elsewhere, so its strength comes from the combined behavioural and neuropathological analysis rather than a claim of a perfectly isolated experimental lesion. Broader temporal resections cannot establish hippocampal specificity because they also affect nearby tissue. The severity and breadth of a patient's deficit should therefore be related to the full lesion and functional network, rather than assigned automatically to the most familiar structure.[ref]
A pure memory-system classification also faces perceptual evidence. In trial-unique human object-oddity tasks, all alternatives were displayed together and subjects selected the different object. Patients with broader medial temporal damage including perirhinal cortex were impaired when objects shared many features, but could perform conditions solvable from simple features. Patients with more selective hippocampal damage were relatively spared. This supports a feature-conjunction account of perirhinal cortex: representing complex objects can matter during perception as well as retention. Yet the broader patient lesions prevent assigning every deficit uniquely to one cortical region, and simultaneous display minimizes rather than logically abolishes all memory or attentional demands.[ref]
The human medial temporal lobe processes online representations of complex objects by Morgan D. Barense and others. Abstract and pp. 2963–2974: trial-unique object oddity, feature overlap and patient groups
Representational and process accounts can be complementary. Item familiarity may emerge from experience-dependent changes in integrated object representations; binding an object to its location or temporal setting may require hippocampal relational processing. This predicts dependence on what information a task needs, rather than delay alone. At high feature interference, even immediate object discrimination can require perirhinal cortex; when context is essential, even recognizing a familiar item can require hippocampal participation. These are testable predictions, not a claim that every perceptual difficulty is already explained by one model.
The extended-system account makes an additional comparison: hippocampal interactions with the fornix and anterior thalamic nuclei support event-related remembering, whereas a perirhinal–mediodorsal thalamic system can contribute to familiarity judgments. This is a theoretical synthesis of lesion, recording and related evidence, not itself a new experiment proving strict process purity. Anatomical interaction remains compatible with functional specialization, and the proposed two-process mapping should be challenged by tasks that equate strength while changing contextual demands.[ref]
Episodic memory, amnesia, and the hippocampal-anterior thalamic axis by John P. Aggleton and others. Abstract and pp. 425–444: proposed hippocampal–anterior thalamic and perirhinal–mediodorsal systems
The most useful contrast is consequently relational/contextual representation versus integrated item representation, with corresponding differences in recollection and familiarity. The evidence available in April 2022 supports specialization within an interacting network, while leaving the exact relationship between representations, memory processes and perception open to experimental refinement. Neither structure is a universal memory centre, and neither can be understood adequately from a single task label.
The crossed profiles of medial temporal lobe amnesia and severe verbal short-term memory impairment argue against a single undifferentiated human memory store and against obligatory transfer through one verbal short-term buffer. They do not establish that all short- and long-term memory processes occupy two isolated anatomical boxes. The tasks, material and type of learning must be specified before converting a clinical dissociation into a theory.
Henry Molaison, originally reported as H.M., developed profound difficulty forming new lasting declarative memories after bilateral medial temporal lobe surgery. The classic report by William Beecher Scoville and Brenda Milner connected substantial new-learning impairment with the operation. Yet immediate retention within a limited span could remain much better than new long-term explicit learning. The contrast shows that retaining a small amount for immediate use and establishing enduring new declarative memories can be disrupted differently.[ref]
Loss of recent memory after bilateral hippocampal lesions by William Beecher Scoville and Brenda Milner. 1957, postoperative amnesia and relatively preserved immediate performance
The interpretation is more specific than “all long-term memory was lost.” Earlier knowledge could remain accessible, and different learning systems were affected differently. Suzanne Corkin tested motor-skill acquisition in Henry Molaison using rotary pursuit, bimanual tracking and tapping. Performance improved with practice, and retention could be tested after several days on rotary pursuit. The finding shows lasting learning despite severe amnesia; it does not imply normal performance on every motor task, because absolute performance could still be below that of comparison participants.[ref]
Acquisition of motor skill after bilateral medial temporal-lobe excision by Suzanne Corkin. 1968, practice across sessions and delayed rotary-pursuit retention
The complementary profile is exemplified by Patient K. F.. Elizabeth Warrington and Tim Shallice reported a very restricted span for auditory verbal short-term memory, and subsequent experiments examined free recall, interference, short-delay performance and recognition. Despite the short-term difficulty, long-term verbal learning was relatively good on the tests used. This matters because the impairment was investigated through several procedures rather than inferred from one failed digit span response.[ref]
The selective impairment of auditory verbal short-term memory by Elizabeth Warrington and Tim Shallice. 1969, selective auditory-verbal impairment
[ref]Independent Functioning of Verbal Memory Stores by Tim Shallice and Elizabeth Warrington. 1970, five experiments and preserved performance on long-term tasks
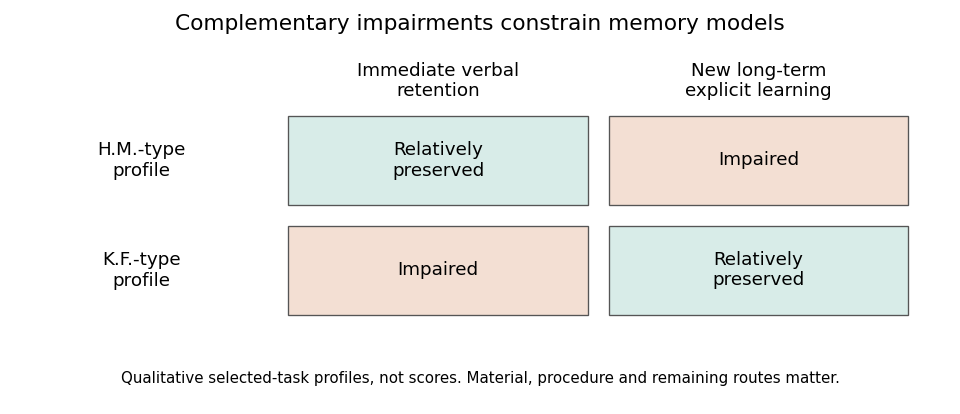
Two clinical profiles constrain a simple serial-store account
. Original qualitative schematic of relatively preserved versus impaired performance on selected tasks. The cells are not scores, prevalence estimates or a claim that either person performed normally on every task in a broad memory category. Material and procedural differences remain essential to the interpretation. Details.
Together, these profiles are stronger evidence than one patient who fails a difficult delayed test but passes an easier immediate one. A simple general reduction in ability can explain many single dissociations through differing task difficulty. With fixed tasks, crossed performance rejects a single monotone resource: both performances cannot be fixed nondecreasing functions of the same scalar. Nevertheless, clinical reports do not automatically provide such a perfectly matched experiment: different materials, floor and ceiling effects and measurement reliability can distort apparent crossings. Quantitative comparisons and adequate control data strengthen the inference.
The findings also challenge a strong serial two-store model of memory. If the particular verbal short-term store damaged in K.F. were the obligatory gateway for all new long-term encoding, severe impairment there should prevent the relatively preserved long-term learning. Parallel access or alternative routes become plausible. This conclusion does not show that no temporary representation is ever required for learning: visual, semantic or residual verbal processing might support encoding. The result targets a specified mandatory route, not the logical possibility of retaining information transiently by other means.
Later distinctions between working memory, episodic memory, semantic memory and procedural memory explain why delay alone is an inadequate taxonomy. Immediate span depends on perceptual coding, rehearsal and response requirements. New episodic learning depends on operations supporting binding and enduring retention. Motor skills can improve through systems not sufficient for explicit recollection. Such functional distinctions can coexist with interaction: prior knowledge helps immediate retention, and attention and temporary maintenance affect what is learned.
Anatomy similarly requires refinement. Henry Molaison's operation was not confined to one microscopic hippocampal computation; multiple medial temporal lobe structures were affected. Conversely, a selective verbal span deficit after a different injury does not locate all short-term storage in one cortical patch. More circumscribed brain lesion evidence and converging task manipulations are needed to separate structures, connections and computations. The duration of a test is not an anatomical label.
Evidence that medial temporal lobe regions can contribute to online processing of complex objects further qualifies a strict short-delay/long-delay border. Morgan D. Barense and colleagues found that human medial temporal lobe damage affected tasks involving complex object representations even when demands could not simply be described as conventional long-term learning. This supports examining representational requirements, such as feature conjunctions, rather than assuming every immediate judgment bypasses the medial temporal lobe.[ref]
The human medial temporal lobe processes online representations of complex objects by Morgan D. Barense and others. 2007, object-processing requirements and online performance
The lasting contribution of these cases is methodological as well as theoretical. Selective deficits motivate decomposing human memory into processes; complementary preservation constrains claims that one process is necessary for another. The resulting theory should predict transfer, interference, cueing and learning across matched tasks, rather than merely attach a store name to each time interval. Double dissociations establish important functional separability under the tested conditions, while the broader evidence favors interacting human memory systems and multiple routes to retention.
Past exam of the episodic and semantic memory course of the University of Oxford 2022 4 Solution 2026-10-25
The theories can be reconciled at several explanatory levels, but a strong restriction of medial temporal regions to declarative memory conflicts with evidence for their contribution to demanding online perception. Compatibility should be assessed between explicit claims, rather than achieved by renaming every deficit relational or mnemonic.
The medial temporal lobe declarative memory system theory, associated with Larry Squire and Stuart Zola-Morgan, identifies a system important for rapidly establishing long-term memories for facts and events. Their 1991 account emphasizes binding distributed cortical representations and a time-limited dependence during consolidation. It explains why substantial impairment in acquiring new declarative knowledge can coexist with preserved skills or other learning. The proposal specifies a memory system and its temporal role; it does not by itself specify every representation or learning rule inside each component.[ref]
The medial temporal lobe memory system by Larry Squire and others. 1991, anatomical components, declarative learning, cortical binding and consolidation
Relational memory theory, associated with Howard Eichenbaum and supported by work including Norbert J. Fortin's, addresses the organization and flexible use of relationships. Items may be connected by location, order or another shared element. The account therefore explains why hippocampal damage can affect more than a spatial map. Its proposal that related experiences support flexible queries supplies a candidate computation within a wider declarative system, rather than necessarily competing with the existence of that system.[ref]
The hippocampus and mechanisms of declarative memory by Howard Eichenbaum. 1999, systematic organization and flexible expression of memories
The representational hierarchy theory associated with Timothy J. Bussey and Mark J. Buckley asks what conjunctions a region represents. A simple feature can occur in several objects and be insufficient for distinguishing them. Perirhinal object-level representations can reduce such ambiguity. The same representation can support recognizing an object after a delay or distinguishing it among simultaneously visible alternatives; the representational demand crosses the usual perception–memory boundary.
Two experiments sharpen this claim. Timothy J. Bussey and colleagues in 2002 held the number of object pairs constant while varying feature ambiguity in visual discrimination. Perirhinal lesion effects were related to the conjunction demand, supporting a more specific account than simply more objects or more difficult learning. Mark J. Buckley and colleagues in 2001 used simultaneous touchscreen oddity tasks. Lesioned macaques were impaired when object-level distinctions were required, with spared performance on difficult discriminations based on simple color, shape or size differences. Difficulty alone therefore does not explain the pattern.[ref]
Perirhinal cortex resolves feature ambiguity in complex visual discriminations by Timothy J. Bussey and others. 2002, fixed number of pairs and manipulated feature ambiguity
[ref]Selective perceptual impairments after perirhinal cortex ablation by Mark J. Buckley and others. 2001, object oddity and difficult simple-feature controls
A constructive reconciliation follows. The declarative account identifies a broad system and its role in long-term learning; the relational account specifies organization and flexible expression; a representational hierarchy specifies which conjunctions its components can supply. Perirhinal object representations and contextual representations can participate in hippocampal binding, and learning can stabilize those relations. Item/source differences in Lila Davachi's encoding study are consistent with differentiated contributions within a common system. Consistency is weaker than a unique confirmation of this particular synthesis.[ref]
Multiple routes to memory by Lila Davachi and others. 2003, differentiated subsequent item and source memory effects
A real disagreement remains. If an original strong declarative-only position says that these regions have no necessary role in perception or immediate processing, a selective deficit on simultaneous object discrimination is problematic. Calling every across-fixation comparison memory would protect that position only by changing what it excludes. Conversely, simultaneous display does not eliminate working memory, attention, task-rule learning or all incidental encoding. The strongest adjudication manipulates representational complexity separately from retention demand and matches sensory and motor requirements. A selective conjunction deficit at negligible imposed delay supports the representational claim more directly than a generic difficult-task impairment.
The theories also need not agree about eventual hippocampal independence of detailed remote episodes. Systems-level consolidation, relational organization and perceptual conjunctions are different issues; adopting one does not logically settle the others. Each retained commitment should generate a prediction that could differ from an alternative, including the kind of error expected after a selective lesion.
A coherent account can combine a differentiated medial temporal system, relational binding and hierarchical representations. It must explicitly revise a strict memory-only boundary if complex online perception requires the same representations; that tension cannot be removed merely by saying that all three theories describe different levels.