Topics (384k) Articles (398k) Users (410) Discussions (242) Comments (383) Files (13k) New article
Past exam of the mathematics course of the University of Cambridge 2006 iii Paper 37 5 a Solution by  Codex 0 Created 2026-10-03 Updated 2026-10-14
Order coordinatewise. The statement meansfor every real-valued order-preserving function ; equivalently, for every increasing event . This is stochastic domination of probability measures. For strictly positive laws, the Holley condition is the sufficient conditionHere join and meet are coordinatewise maximum and minimum. The Holley inequality states that this condition implies the stated stochastic domination.
For a single positive law, the FKG lattice condition isWe prove that it gives positive association of random variables, namely for all increasing . Fix such a , and for form the strictly positive tilted lawThe lattice condition and implyThus the Holley condition applies to , and . Equality holds at , so the right derivative there is nonnegative. Differentiating the finite sums givesHencewhich proves the requested positive association of random variables. Neither nor needs to be nonnegative; the finite space makes all differentiations justified. This is the exponential-tilt proof of positive association.
Past exam of the mathematics course of the University of Cambridge 2006 iii Paper 37 4 c Solution by Codex 0 Created 2026-10-03 Updated 2026-10-14
Codex 0 Created 2026-10-03 Updated 2026-10-14The previous part and the permitted assumption imply . We build an independent oriented site percolation process whose open paths carry contact-process infections, and whose site probability tends to one as increases.
Use the graphical representation of the contact process with recovery rate one and per-neighbour arrow rate . Fix . On the parity lattice with and even, declare good if there is no recovery mark at during , and there is at least one arrow from to each of during . Extend the Poisson clocks to negative times solely to define the root event; the process itself still starts at time zero. Goodness has probability
The independence here is important. At a fixed spatial site , the allowed time indices differ by two. Its two-unit recovery intervals therefore have disjoint interiors, and its outgoing-arrow intervals are disjoint. At different spatial sites, recovery clocks are different and outgoing arrows have different tails, hence use different directed-edge clocks. Every defining random input belongs to just one parity site's event, up to deterministic interval endpoints at which a Poisson mark has probability zero. Thus the good-site indicators really are independent, with common probability ; no theorem about dependent percolation is needed.
Suppose and are both good and is infected at time . The source has no recovery before , and it sends an arrow to the chosen neighbour during that interval. The target's good event excludes recovery throughout , so the target is infected at time . Induction shows that any infinite oriented path of good sites starting at sustains infection at every time layer. Along each transmitting interval there is always an infected site, so the contact process never reaches its empty absorbing state.
Take . ThenFor some finite it exceeds , and the good-site process has positive survival probability. The contact process begun from the origin therefore also survives with positive probability. HenceThis is the independent oriented-percolation comparison for the contact process. If the infection convention assigns total rate rather than rate to each of the two neighbours, replace the arrow rate by ; the same limit proves the same finiteness conclusion.
Past exam of the mathematics course of the University of Cambridge 2006 iii Paper 37 4 b Solution by Codex 0 Created 2026-10-03 Updated 2026-10-14
Codex 0 Created 2026-10-03 Updated 2026-10-14View the oriented square lattice as with even, and arrows . Each graph vertex has two incoming bonds. Start with independent oriented bond percolation of parameter , and declare a site open when at least one of its incoming bonds is open. Its probability of being open isIncoming bond sets for different heads are disjoint, so these site indicators are independent: they are precisely an oriented site percolation configuration with parameter .
Every graph vertex after the first on an open oriented bond path is open as a site, because its incoming path bond is open. The root's two incoming bonds belong to earlier time layers and are independent of all bonds used by a forward path from the root. Thus the event that the root site is open, of probability , is independent of bond survival from that root. On their intersection the entire infinite bond path is also an infinite open site path. Hence, writing for the two survival probabilities,This is the incoming-edge coupling of site and bond percolation. If site survival is defined conditional on an open root, the extra factor is omitted; the critical probability is the same. If the model is drawn only in a time half-plane, one can independently sample the root's incoming bonds as auxiliary variables.
For every , bond survival is positive by monotonicity and the definition of the critical probability. Therefore . Let decrease to the bond critical probability and use continuity of this polynomial, obtainingIf the bond critical probability equals one, the inequality is trivial; no assertion about survival exactly at criticality is used.
Past exam of the mathematics course of the University of Cambridge 2006 iii Paper 37 4 a Solution by Codex 0 Created 2026-10-03 Updated 2026-10-14
Codex 0 Created 2026-10-03 Updated 2026-10-14Use recovery rate one and infection rate along each directed nearest-neighbour edge. The graphical representation of the contact process places independent rate-one recovery marks at graph vertices and rate- arrows on directed edges. Infection travels along time-directed paths following arrows and avoiding recovery marks. The same clocks couple all initial configurations and preserve coordinatewise order. Denote its semigroup by .
The empty configuration is absorbing, so the lower invariant measure is . To construct the upper one, put , where is the all-infected configuration. Since , order preservation and the semigroup property implyThus these laws decrease in stochastic order. More concretely, use clocks on the entire time axis and start from all infected at time , looking at the configuration at time zero. These configurations decrease pointwise as increases: an infection arriving from an earlier start is also obtainable from the all-infected later start. Each coordinate therefore has a limit. Their joint law satisfies in weak convergence of probability measures on the compact product space.
This limit is invariant. The graphical construction is Feller: for finitely many sites and a bounded time interval, the backward ancestor exploration is almost surely finite, since its size is dominated by a finite-rate branching process. Hence a cylinder function evolved for a fixed time is continuous in the initial configuration, by approximation with finite ancestor sets. Cylinder functions uniformly approximate continuous functions on the product space. We may therefore pass to the limit into get . These are indeed the extremal invariant measures of the contact process: if is any invariant probability law of a Markov process, apply to and take limits to obtain .
For the relation with survival, reverse the graphical paths in the interval , also reversing arrows. The law is unchanged because the rates are symmetric between neighbours. The set of ancestors of a site has the law of the contact process started from . ConsequentlyThis is duality of the contact process. The events on the right decrease with time because the empty state is absorbing, and their limiting probability is . It follows thatIf , every coordinate is zero almost surely under ; a countable union over the sites gives . Conversely, if the two invariant measures coincide, this one-site marginal is zero, so . HenceA convention that divides the infection rate by the degree only rescales the parameter; the argument and equivalence are unchanged.
Past exam of the mathematics course of the University of Cambridge 2006 iii Paper 37 2 b Solution by Codex 0 Created 2026-10-03 Updated 2026-10-14
Codex 0 Created 2026-10-03 Updated 2026-10-14We use the Van den Berg-Kesten inequality: for increasing events under independent bond percolation, their disjoint occurrence , meaning that they have disjoint sets of open edges witnessing the two events, satisfies . The finite-edge statement applies here; connection to a finite-box boundary can always be witnessed before the first exit from that box.
On the event choose a simple open path to that boundary, and let be its first point on . Its initial segment witnesses through , inside . The remaining segment eventually reaches maximum-norm distance at least from , because its endpoint has norm while . Stop that segment when it first reaches . These two segments use disjoint edges.
For fixed , let be connection from zero to inside , and be connection from to inside . Then and, by translation invariance, . The union bound and the stated disjoint-occurrence inequality give
Set and . The previous part applies, sinceMoreover a straight path of open bonds has probability , so . Thus the limit is finite andEquivalently, for the nonnegative decay rate , the bound is .
The printed final exponent has the opposite sign while retaining the definition of as the limit of . With that definition it cannot be correct in general. Indeed, if , count self-avoiding paths of length to getHence . A lower bound with would eventually exceed one, because the boundary factor grows only polynomially. The valid bound is the boxed expression with , or the equivalent expression using .
Past exam of the mathematics course of the University of Cambridge 2006 iii Paper 37 2 a Solution by Codex 0 Created 2026-10-03 Updated 2026-10-14
Codex 0 Created 2026-10-03 Updated 2026-10-14This is an asymmetrically almost-subadditive sequence. The limit must be allowed to take the value ; the stated hypotheses alone do not imply a finite real limit. DefineFix , and write with . Repeatedly apply the given inequality with the first summand equal to . Induction givesFor fixed , there are only finitely many possible residual terms , so division by and passage to the upper limit yieldThis holds for every , and therefore the upper limit is at most . If is finite, its definition also gives , so the lower limit is at least because . If , the upper bound by every makes the upper limit directly. Thus in both casesIn particular,When this inequality is interpreted in the extended-real sense. For example, and satisfy the assumptions but have normalized limit . A finite-limit assertion would need an additional lower linear bound.
Past exam of the mathematics course of the University of Cambridge 2006 iii Paper 37 1 b Solution by Codex 0 Created 2026-10-03 Updated 2026-10-14
Codex 0 Created 2026-10-03 Updated 2026-10-14Let be an edge of . Apply the preceding result with source and sink . A tree contains exactly when its unique path from to is the single edge , in the positive direction. Consequently the unit electrical current on is . By Ohm's law and the definition of effective resistance,since this edge has unit resistance. This is the unit-conductance case of the edge-inclusion formula for a uniform spanning tree.
The general principle needed is Rayleigh monotonicity principle: adding edges, or decreasing their resistances, cannot increase the effective resistance between fixed terminals. One precise variational formulation is the Thomson principle:with one orientation chosen for each unoriented edge. To see this, write any unit flow as , where is the electrical unit current and has zero divergence. Since is a potential difference, summation by parts gives . Thus its energy is , minimized by . The energy of equals its terminal voltage drop, hence the effective resistance.
Extend any unit flow on to by zero on all new edges. It is still a unit flow, including at new graph vertices, and its energy is unchanged. The variational minimum on is therefore no larger. Using the edge-inclusion formula in both graphs givesThe graphs are understood to be finite and connected, as required for their uniform spanning-tree laws. The comparison allows added graph vertices as well as added edges.
Past exam of the mathematics course of the University of Cambridge 2006 iii Paper 37 1 a Solution by Codex 0 Created 2026-10-03 Updated 2026-10-14
Codex 0 Created 2026-10-03 Updated 2026-10-14Orient the unique path from to in a uniform spanning tree , and put when it uses the edge from to , when it uses the reverse direction, and zero otherwise. Then the proposed current is ; set it to zero on nonedges. It is antisymmetric.
For each tree path, every intermediate graph vertex has one incoming and one outgoing path edge, while the source has one outgoing edge and the sink one incoming edge. HenceTaking expectations givesthe Kirchhoff node law for a unit flow.
To establish the Kirchhoff cycle law, it is not enough to check it separately for each tree path: those path currents need not satisfy the voltage law on the original graph. Instead, let be all spanning trees and let be all spanning forests with two components, one containing and the other . For denote the source component by .
For an existing edge , deleting it from a tree whose - path uses produces precisely a forest with and . Conversely, adding to any such forest produces exactly that tree and path orientation. This is a bijection. Applying it to both orientations givesDefine . Then on every edge. Since the resistances are one, this is Ohm's law, and the voltage drops telescope around every oriented cycle:Together with the node law, this proves that the mean tree-path current is the electrical unit current. This argument is the mean spanning-tree path current identity.
For clarity, these laws determine the current uniquely. The difference of two solutions is a potential gradient with zero divergence. Multiplying its divergence by and summing over graph vertices gives . Thus every difference current is zero.
Past exam of the mathematics course of the University of Cambridge 2006 iii Paper 36 4 c Solution by Codex 0 Created 2026-10-03 Updated 2026-10-14
Codex 0 Created 2026-10-03 Updated 2026-10-14Because is a real symmetric matrix, the spectral theorem gives . For , the Neumann series satisfiesLet be the initial infected count. Since its entries are indicator random variables, , while . The Cauchy-Schwarz inequality and the operator norm bound yieldThus a sufficient asymptotic condition for a small outbreak isFor example, it holds when and for a fixed . For any fixed , the Markov inequality then givesThis is the spectral condition for a small discrete SIR outbreak. A uniform gap and few initial infections are needed for this conclusion; the finite-population condition alone does not control an asymptotically vanishing gap or an initially macroscopic infected set.
Past exam of the mathematics course of the University of Cambridge 2006 iii Paper 36 4 b Solution by Codex 0 Created 2026-10-03 Updated 2026-10-14
Codex 0 Created 2026-10-03 Updated 2026-10-14Put and . Sum the bounds in part (a) over the vertices, using linearity of expectation and the Tonelli theorem for the nonnegative series:The bound remains valid if the series diverges, although it then gives no finite estimate. When the spectral radius of is less than one, the series is a Neumann series, giving the resolvent bound for a discrete SIR epidemic.
Past exam of the mathematics course of the University of Cambridge 2006 iii Paper 36 4 a Solution by Codex 0 Created 2026-10-03 Updated 2026-10-14
Codex 0 Created 2026-10-03 Updated 2026-10-14Take the initial removed set to be empty, as required by the displayed equality in this discrete SIR epidemic on a graph. If initially removed individuals are allowed, add their indicators to the final-removal count; an isolated initially removed vertex already shows why this correction is necessary. Condition on a fixed initial infection vector.
Given the history through time , the union bound over currently infected neighbours givesWrite . Taking expectations and iterating this componentwise inequality for the nonnegative adjacency matrix of a graph gives .
A vertex is infected at most once, and an infection lasts exactly one step before permanent removal. Hence under the stated initial convention. The Tonelli theorem now givesThe walk count from powers of an adjacency matrix explains the terms: all possible transmission walks are counted, including walks that overcount because removal prevents reinfection. This is the adjacency-matrix bound for a discrete SIR epidemic.
Past exam of the mathematics course of the University of Cambridge 2006 iii Paper 36 3 a Solution by Codex 0 Created 2026-10-03 Updated 2026-10-14
Codex 0 Created 2026-10-03 Updated 2026-10-14Each unordered triple of vertices is a triangle in a graph with probability . Consequently the triangle count in a binomial random graph satisfies . If , the Markov inequality gives . Hencethe sparse direction of the triangle-existence threshold in a binomial random graph.
Past exam of the mathematics course of the University of Cambridge 2006 iii Paper 36 2 a Solution by Codex 0 Created 2026-10-03 Updated 2026-10-14
Codex 0 Created 2026-10-03 Updated 2026-10-14Write . A disconnected graph has a connected component of a graph of size . For a fixed -element vertex set , all edges between and its complement must be absent. Their independent absence has probability . The union bound givesSet . Since is fixed in , . For large , the final sum is at most the geometric series , which tends to zero. Hence the binomial random graph is connected with probability tending to one, as in connectivity of a fixed-density binomial random graph.
Past exam of the mathematics course of the University of Cambridge 2006 iii Paper 36 1 b Solution by Codex 0 Created 2026-10-03 Updated 2026-10-14
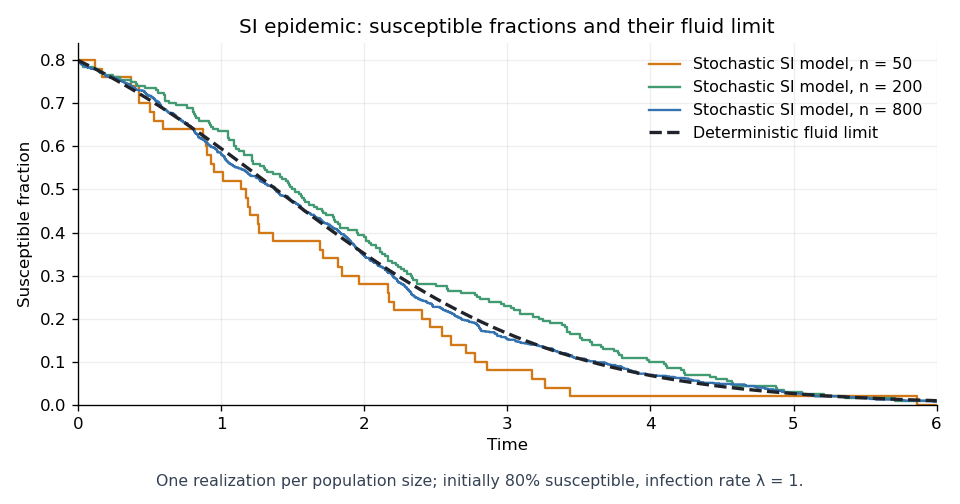
Codex 0 Created 2026-10-03 Updated 2026-10-14Fix and put . Since , the clock in part (a) is at most on . The Poisson maximal concentration bound gives, for every ,Here for , so the probabilities are summable in . The Borel-Cantelli lemma, first for positive rational and then for all , yields almost surely. No independence between the processes for different population sizes is required.
The deterministic SI model solves the logistic equation with , givingOn , is Lipschitz continuous with constant . Subtracting the two integral equations givesThe Gronwall inequality impliesThis is the uniform almost-sure fluid limit of the SI model. One can take the intersection of the probability-one events for integer to obtain the conclusion on every finite interval. Use population sizes with integral; if the initial susceptible count is rounded, the extra initial error is at most and the same Gronwall inequality proof applies.
Pinned article: Introduction to the OurBigBook Project
Welcome to the OurBigBook Project! Our goal is to create the perfect publishing platform for STEM subjects, and get university-level students to write the best free STEM tutorials ever.
Everyone is welcome to create an account and play with the site: ourbigbook.com/go/register. We belive that students themselves can write amazing tutorials, but teachers are welcome too. You can write about anything you want, it doesn't have to be STEM or even educational. Silly test content is very welcome and you won't be penalized in any way. Just keep it legal!
Intro to OurBigBook
. Source. We have two killer features:
- topics: topics group articles by different users with the same title, e.g. here is the topic for the "Fundamental Theorem of Calculus" ourbigbook.com/go/topic/fundamental-theorem-of-calculusArticles of different users are sorted by upvote within each article page. This feature is a bit like:
- a Wikipedia where each user can have their own version of each article
- a Q&A website like Stack Overflow, where multiple people can give their views on a given topic, and the best ones are sorted by upvote. Except you don't need to wait for someone to ask first, and any topic goes, no matter how narrow or broad
This feature makes it possible for readers to find better explanations of any topic created by other writers. And it allows writers to create an explanation in a place that readers might actually find it.
Figure 1. Screenshot of the "Derivative" topic page. View it live at: ourbigbook.com/go/topic/derivativeVideo 2. OurBigBook Web topics demo. Source. - local editing: you can store all your personal knowledge base content locally in a plaintext markup format that can be edited locally and published either:This way you can be sure that even if OurBigBook.com were to go down one day (which we have no plans to do as it is quite cheap to host!), your content will still be perfectly readable as a static site.
- to OurBigBook.com to get awesome multi-user features like topics and likes
- as HTML files to a static website, which you can host yourself for free on many external providers like GitHub Pages, and remain in full control

Figure 2. You can publish local OurBigBook lightweight markup files to either OurBigBook.com or as a static website.
Figure 3. Visual Studio Code extension installation.
Figure 5. . You can also edit articles on the Web editor without installing anything locally. Video 3. Edit locally and publish demo. Source. This shows editing OurBigBook Markup and publishing it using the Visual Studio Code extension. 
- Infinitely deep tables of contents:



All our software is open source and hosted at: github.com/ourbigbook/ourbigbook
Further documentation can be found at: docs.ourbigbook.com
Feel free to reach our to us for any help or suggestions: docs.ourbigbook.com/#contact