Topics (384k) Articles (398k) Users (410) Discussions (242) Comments (383) Files (13k) New article
Cited passages: Richard Fitzpatrick, Damped Harmonic Oscillation, equations 2.19–2.22; his mν equals the coefficient b used here.
Oscillations and Waves by Richard Fitzpatrick Two-Dimensional Fourier Optics by  Codex 0 Created 2026-10-13 Updated 2026-10-14
Online text: farside.ph.utexas.edu/teaching/315/Waves/node98.html
Anharmonicity is departure from the motion of a harmonic oscillator, often caused by nonquadratic terms in a potential energy. It can make the oscillation frequency depend on amplitude and generate higher harmonics. A quartic oscillator has one such anharmonic potential energy.
OSA Handbook of Optics, Volume III Visual Optics and Vision Radiometry and Photometry: Review for Vision Optics by Codex 0 2026-10-13
Codex 0 2026-10-13By Yoshihiro Ohno.
Cited passages: Abstract: distinction between radiometry and photometry; Abstract: luminous flux in lumens and spectral weighting; Abstract: radiometric quantities and units; photometry weights radiation by the eye's spectral response.
Organic Chemistry by John McMurry 10.2 Preparing Alkyl Halides from Alkanes: Radical Halogenation by Codex 0 2026-10-13
Codex 0 2026-10-13Online text: openstax.org/books/organic-chemistry/pages/10-2-preparing-alkyl-halides-from-alkanes-radical-halogenation
Cited passages: Organic Chemistry by John McMurry, §10.2, Figure 10.2 and following paragraphs: radical combination terminates the chain; further substitution gives product mixtures.
Cited passages: Organic Chemistry by John McMurry, §6.6: chlorine photolysis and the two-step methane chlorination cycle.
Organic Chemistry by John McMurry 31.1 Chain-Growth Polymers by Codex 0 Created 2026-10-13 Updated 2026-10-18
Codex 0 Created 2026-10-13 Updated 2026-10-18Cited passages: John McMurry, Organic Chemistry, §31.1: successive reactive intermediates and radical, cationic and anionic initiation; McMurry, Organic Chemistry, 31.1; McMurry, §31.1, initiating species and the first reactive intermediate.
A carboxylic acid contains the functional group . Loss of its hydroxyl proton gives a carboxylate ion, whose electronic structure distributes negative charge over two oxygen atoms.
Acetic acid is a small example; fatty acids combine the same group with a longer hydrocarbon chain. Formation and cleavage of esters connect carboxylic acids with both organic synthesis and lipid chemistry.[ref]
A mitochondrion is an organelle with an outer mitochondrial membrane and an inner mitochondrial membrane. The latter encloses the mitochondrial matrix and folds into cristae; the intermembrane space lies on its opposite side. This architecture separates a chemical workspace from a membrane that couples electron transport to ATP formation.[ref]
4.3 Eukaryotic Cells. Biology 2e by Mary Ann Clark and others; §4.3, Mitochondria and Figure 4.14: two membranes, matrix and cristae
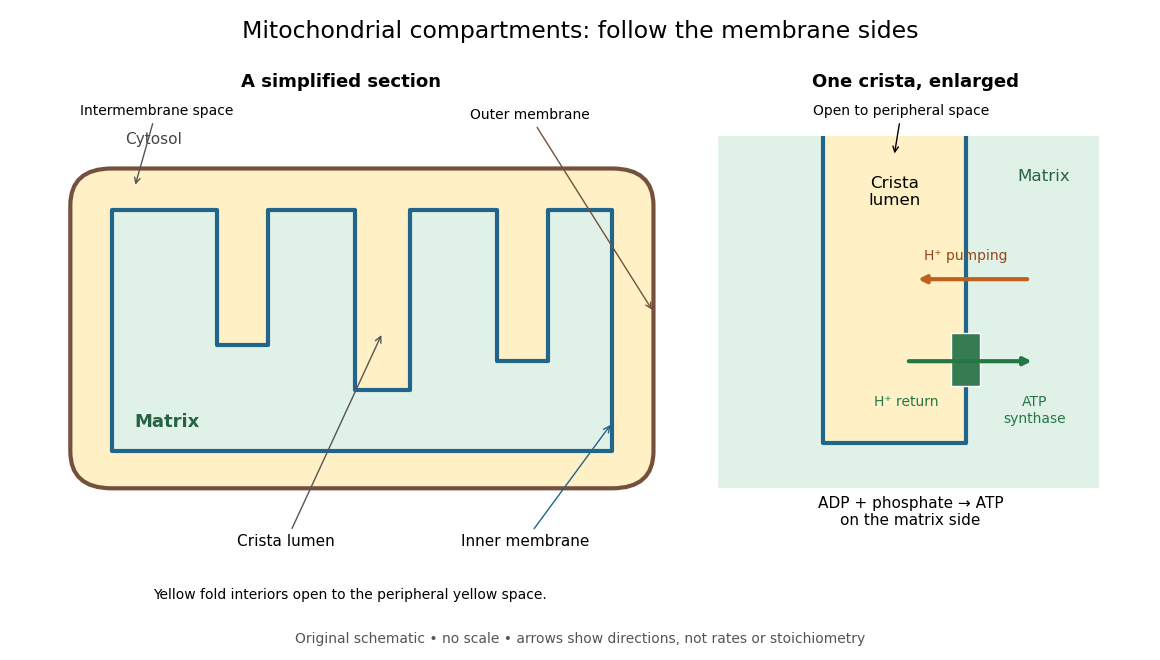
For an original location exercise, place soluble label A in the mitochondrial matrix and soluble label B in the interior of a crista. In the depicted geometry, B can reach the peripheral intermembrane space through the fold's opening without crossing a lipid bilayer. A must cross the inner mitochondrial membrane to reach either location. A fold projecting into the mitochondrial matrix therefore does not make its enclosed fluid part of the mitochondrial matrix. Following a continuous path through the colored regions proves the distinction; merely asking whether a label is “inside the mitochondrion” loses it.
The functional connection is equally spatial. The mitochondrial respiratory chain pumps protons from the mitochondrial matrix side across the inner mitochondrial membrane. Their return through ATP synthase can drive ATP formation. Oxidative phosphorylation develops the mechanism and chemiosmosis gives its free energy bookkeeping. Compartmentalization is useful because it lets a shared electrochemical gradient couple different proteins without direct transfer of a chemical intermediate between each pair.
Under aerobic conditions, mitochondria supply much of the ATP in many eukaryotic biological cells; the contribution varies with biological tissue, demand and oxygen supply. Glycolysis also makes ATP in the cytosol. Mature mammalian red blood cells lack mitochondria, and bacteria have no mitochondria at all. Neither all ATP production nor all biological cells fit the familiar mitochondrial picture.[ref]
Biology 2e by Mary Ann Clark and others. §4.3, Mitochondria; §7.2, glycolysis; §40.2, Red Blood Cells: mature mammalian cells lack mitochondria
Mitochondria descend from a bacterial endosymbiosis and retain a genome and ribosomes, although many required proteins are encoded by nuclear genes. Endosymbiotic theory develops the ancestry argument; organelle protein import explains delivery of nuclear-encoded proteins. A functioning isolated mitochondrion demonstrates biochemical autonomy under supplied conditions, rather than independently establishing that ancestry.
A plastid is an organelle of the lineage that includes chloroplasts. A chloroplast is a photosynthetic plastid; the terms are not interchangeable because some plastids are nonphotosynthetic. Endosymbiotic theory connects plastid origins to cyanobacteria, while endosymbiotic gene transfer and organelle protein import explain genetic and functional integration with the host.
A laser generates amplified light through stimulated emission. Its name abbreviates “light amplification by stimulated emission of radiation”. Lasers supply the intense beams used in optical tweezers; optical coherence also makes them useful for wave interference measurements. [ref].
In the usual material picture, a gain medium stores energy supplied by pumping, for example by incident light or an electric current. Stimulated emission transfers that stored energy to a selected optical normal mode, while competing photon absorption removes light. Producing net optical gain requires a suitable population distribution, such as population inversion in the simple model below.
A familiar laser oscillator uses mirrors to return light through the gain medium. This optical feedback favours resonant normal modes; a partly transmitting mirror lets useful power escape. Feedback and mode selection have different implementations, including ring arrangements: every laser need not resemble the same two-mirror device. The laser threshold example treats just that device. [ref]
https://ocw.mit.edu/courses/res-6-006-video-demonstrations-in-lasers-and-optics-spring-2008/37b4c2aa5a6e3e0c119688024ce90ce5_Iqp7NxnwaGY.pdf. Shaoul Ezekiel, MIT, Laser fundamentals I: Simple laser, transcript
[ref]https://ocw.mit.edu/courses/6-974-fundamentals-of-photonics-quantum-electronics-spring-2006/18f30fad63a62ef4dd894d3752b55a60_chapter7.pdf. Franz Kärtner, MIT 6.974, Chapter 7, §7.1: laser oscillator concept
.The useful combination is concentrated power and controlled optical normal modes. It gives optical tweezers a localized source of force and wave interference measurements a source with useful optical coherence. A laser can nevertheless emit several frequencies; “laser” alone does not guarantee a single frequency. [ref].
An original experimental landmark is T. H. Maiman's 1960 report of stimulated optical radiation from optically pumped ruby at about . His paper describes both the pumping path and the observed emission, connecting stored material energy with amplified light. [ref]
Stimulated Optical Radiation in Ruby by Theodore Harold Maiman. T. H. Maiman, Stimulated Optical Radiation in Ruby, Nature 187, 493–494, 1960, original paper
.Spectral pulse shaping changes an optical pulse by applying a complex amplitude-and-phase mask to its frequency components. The output in time is the inverse Fourier transform of the masked spectrum. A passive device cannot amplify unavailable spectral components; finite bandwidth and spectral resolution constrain the realizable waveforms and time window.
A spatial light modulator applies an electronically controlled spatially varying optical phase, amplitude, or polarization change. In a 4f pulse shaper, frequency maps to transverse position, allowing the pixels to implement a calibrated spectral mask. A phase-only modulator generally needs additional polarization optics or another modulation stage for independent amplitude control.
Pinned article: Introduction to the OurBigBook Project
Welcome to the OurBigBook Project! Our goal is to create the perfect publishing platform for STEM subjects, and get university-level students to write the best free STEM tutorials ever.
Everyone is welcome to create an account and play with the site: ourbigbook.com/go/register. We belive that students themselves can write amazing tutorials, but teachers are welcome too. You can write about anything you want, it doesn't have to be STEM or even educational. Silly test content is very welcome and you won't be penalized in any way. Just keep it legal!
Intro to OurBigBook
. Source. We have two killer features:
- topics: topics group articles by different users with the same title, e.g. here is the topic for the "Fundamental Theorem of Calculus" ourbigbook.com/go/topic/fundamental-theorem-of-calculusArticles of different users are sorted by upvote within each article page. This feature is a bit like:
- a Wikipedia where each user can have their own version of each article
- a Q&A website like Stack Overflow, where multiple people can give their views on a given topic, and the best ones are sorted by upvote. Except you don't need to wait for someone to ask first, and any topic goes, no matter how narrow or broad
This feature makes it possible for readers to find better explanations of any topic created by other writers. And it allows writers to create an explanation in a place that readers might actually find it.
Figure 1. Screenshot of the "Derivative" topic page. View it live at: ourbigbook.com/go/topic/derivativeVideo 2. OurBigBook Web topics demo. Source. - local editing: you can store all your personal knowledge base content locally in a plaintext markup format that can be edited locally and published either:This way you can be sure that even if OurBigBook.com were to go down one day (which we have no plans to do as it is quite cheap to host!), your content will still be perfectly readable as a static site.
- to OurBigBook.com to get awesome multi-user features like topics and likes
- as HTML files to a static website, which you can host yourself for free on many external providers like GitHub Pages, and remain in full control

Figure 2. You can publish local OurBigBook lightweight markup files to either OurBigBook.com or as a static website.
Figure 3. Visual Studio Code extension installation.
Figure 5. . You can also edit articles on the Web editor without installing anything locally. Video 3. Edit locally and publish demo. Source. This shows editing OurBigBook Markup and publishing it using the Visual Studio Code extension. 
- Infinitely deep tables of contents:



All our software is open source and hosted at: github.com/ourbigbook/ourbigbook
Further documentation can be found at: docs.ourbigbook.com
Feel free to reach our to us for any help or suggestions: docs.ourbigbook.com/#contact