Topics (384k) Articles (398k) Users (410) Discussions (242) Comments (383) Files (13k) New article

A membrane channel whose opening depends on membrane potential. Regenerative activation and subsequent inactivation or opposing currents help produce an action potential.
A reversal potential is a membrane potential at which a specified open ion channel, or specified combination of ion channels, carries zero net electric current, with the surrounding conditions fixed; the electric current changes sign across that voltage. Specifying which current matters: an individual ion contribution and a sum of several contributions can reverse at different voltages. Zero net electric current does not mean that all ions have stopped moving. See Purves et al., Neuroscience, 2nd edition (2001): reversal of a mixed-ion channel current.
Throughout these examples, membrane potential is , and conventional current is inward-positive. Positive electric current corresponds to net positive electric charge entering or net negative electric charge leaving. Negative electric current corresponds to the reverse charge transfer. A convenient Ohmic approximation iswhere is the available electrical conductance. For fixed , gives positive electric current, gives zero, and gives negative electric current; the line has slope . If , the modeled pathway carries zero electric current at every voltage: closing it does not locate its reversal potential. 3.1 Synapses (§3.1: conductance-based synaptic current) uses outward-positive ; the formula here reverses that sign to match this wiki's inward-positive convention.
For the stipulated single-pathway example from ion channel, and giveThe open ion channel carries zero net electric current at even though remains positive. Near that point a change of membrane potential changes the electric current, which is why zero current at one voltage does not make an open pathway electrically irrelevant; see shunting inhibition.
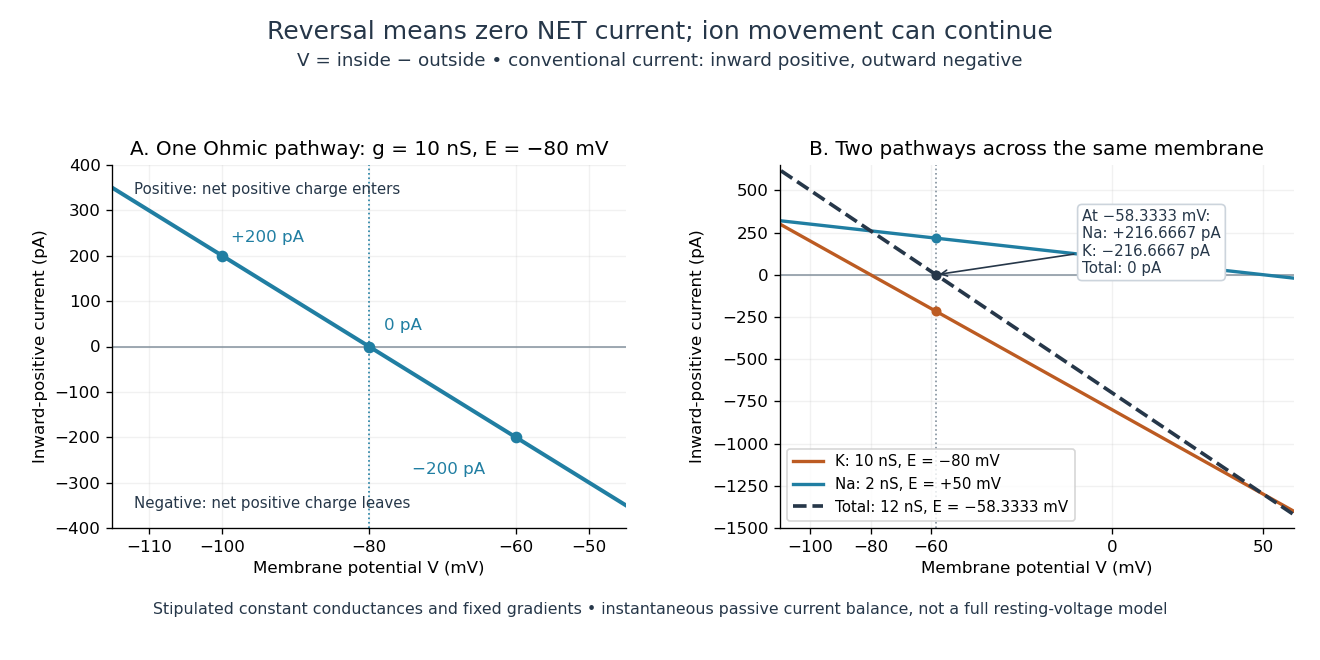
Inward-positive electric current: one reversal and two-channel cancellation
. Original computed curves for stipulated constant electrical conductances and fixed reversal potentials. Left: , . Right: a potassium pathway with , and a sodium pathway with , . Their net electric current vanishes at while both individual electric currents remain nonzero. These are model values, not empirical measurements. Details.For an ion channel passing only one ion species by passive transport, its reversal potential can equal that species' Nernst equilibrium potential, where the chemical and electrical contributions to electrochemical potential balance. At that thermodynamic equilibrium, passage in both directions can continue with no net transport. For an ion channel admitting several ion species, opposing contributions can cancel while each species continues to have net transport. Such a reversal potential is not generally any one species' Nernst equilibrium potential. See the Purves reference above.
To work out that cancellation explicitly, put two Ohmic ion channel populations across the same cell membrane. Stipulate constant electrical conductances and fixed reversal potentials:The potassium and sodium contributions add because both pathways experience the same membrane potential:Thus . This weighted mean follows simply by expanding and regrouping the two current terms; it assumes additive Ohmic contributions and a positive total electrical conductance. At , the inward-positive individual electric currents areThe potassium contribution is outward and the sodium contribution inward. Equal and opposite electric currents give ; neither pathway has stopped transporting its ions. The calculation treats two distinct pathways. Applying it to one mixed-species ion channel would additionally require a justified decomposition into independent Ohmic contributions; a general mixed-channel reversal potential cannot be obtained by assuming those hypotheses silently.
This is an instantaneous balance of the specified passive electric currents. It would be the stationary voltage of a passive capacitance model containing only these constant pathways and no applied electric current, but it is not a complete prediction of a living cell's resting membrane potential. Other electric currents, voltage-dependent gating, and pumps involved in active transport can matter. Pumps that transfer net electric charge are electrogenic and contribute their own electric current. See Purves et al.: functional properties of the sodium/potassium pump.
The toy model holds ion concentrations and therefore the stipulated reversal potentials fixed. Continuing inward sodium and outward potassium transport would change finite reservoirs unless active transport or external control maintained them. Transport can be a small fraction of the reservoir's ions over a short interval, making fixed concentrations a useful approximation; it is not a claim that the reservoirs never change. See Gerstner et al., Neuronal Dynamics (2014), §2.1: equilibrium potentials, channel currents and maintained gradients.
A reversal potential makes the effect of opening an ion channel predictable from the present membrane potential. The same open pathway can carry inward or outward electric current as crosses its reversal potential. The two-pathway example reveals a particularly useful distinction: zero net charge transfer can coexist with continuing exchange of different substances. That distinction connects membrane transport to electric current measurements without mistaking electrical balance for thermodynamic equilibrium.
Hyperpolarization makes a neuronal membrane potential more negative relative to the exterior. It is a voltage description; inhibition need not produce hyperpolarization, as shunting inhibition illustrates.
For a negative neuronal membrane potential, depolarization raises it toward zero or beyond, making the interior less negative relative to the exterior. This describes a voltage change, not necessarily increased action potential generation; see the depolarizing inhibition example under synaptic potential.
Ploidy counts sets of chromosomes; DNA amount counts material. Let be the number of chromosomes in one complete set and the DNA amount of one unreplicated set. For the ordinary diploid model, read each row per completed cell nucleus, not as a total across all products:
| Stage | Ploidy | DNA amount | Chromosome organization |
|---|---|---|---|
| Before DNA replication | Two unreplicated sets | ||
| After DNA replication | Two sets; each chromosome has two sister chromatids | ||
| After meiosis I | One replicated set | ||
| After meiosis II | One unreplicated set |
In the illustrated example, the starting biological cell has four chromosomes. DNA replication gives eight chromatids, organized into four replicated chromosomes. Each product of meiosis I has two replicated chromosomes, hence four chromatids; each final product has two unreplicated chromosomes. Across completed products, after meiosis I and after meiosis II: division redistributes the replicated DNA. A haploid cell nucleus can therefore have without becoming diploid.
The second division of meiosis separates sister chromatids, without an intervening round of DNA replication.
The first division of meiosis separates replicated homologous chromosomes; their sister chromatids remain associated.
Cited passages: Hunter, Measure Theory, Definition 7.4: the L-infinity norm; Hunter, Measure Theory, Definitions 7.1 and 7.4: Lp spaces and norms; Hunter, Measure Theory, Definitions 7.1, 7.3–7.4: almost-everywhere equivalence and essential bounds; Hunter, Measure Theory, §7.4, Lemma 7.9, pp. 81–82, and Theorem 7.10, pp. 82–83: norm summability and completeness.
Optimization with no additional optimization constraints on the chosen variable domain. At an interior local extremum of a differentiable function, the first-order optimality condition is .
Pinned article: Introduction to the OurBigBook Project
Welcome to the OurBigBook Project! Our goal is to create the perfect publishing platform for STEM subjects, and get university-level students to write the best free STEM tutorials ever.
Everyone is welcome to create an account and play with the site: ourbigbook.com/go/register. We belive that students themselves can write amazing tutorials, but teachers are welcome too. You can write about anything you want, it doesn't have to be STEM or even educational. Silly test content is very welcome and you won't be penalized in any way. Just keep it legal!
Intro to OurBigBook
. Source. We have two killer features:
- topics: topics group articles by different users with the same title, e.g. here is the topic for the "Fundamental Theorem of Calculus" ourbigbook.com/go/topic/fundamental-theorem-of-calculusArticles of different users are sorted by upvote within each article page. This feature is a bit like:
- a Wikipedia where each user can have their own version of each article
- a Q&A website like Stack Overflow, where multiple people can give their views on a given topic, and the best ones are sorted by upvote. Except you don't need to wait for someone to ask first, and any topic goes, no matter how narrow or broad
This feature makes it possible for readers to find better explanations of any topic created by other writers. And it allows writers to create an explanation in a place that readers might actually find it.
Figure 1. Screenshot of the "Derivative" topic page. View it live at: ourbigbook.com/go/topic/derivativeVideo 2. OurBigBook Web topics demo. Source. - local editing: you can store all your personal knowledge base content locally in a plaintext markup format that can be edited locally and published either:This way you can be sure that even if OurBigBook.com were to go down one day (which we have no plans to do as it is quite cheap to host!), your content will still be perfectly readable as a static site.
- to OurBigBook.com to get awesome multi-user features like topics and likes
- as HTML files to a static website, which you can host yourself for free on many external providers like GitHub Pages, and remain in full control

Figure 2. You can publish local OurBigBook lightweight markup files to either OurBigBook.com or as a static website.
Figure 3. Visual Studio Code extension installation.
Figure 5. . You can also edit articles on the Web editor without installing anything locally. Video 3. Edit locally and publish demo. Source. This shows editing OurBigBook Markup and publishing it using the Visual Studio Code extension. 
- Infinitely deep tables of contents:



All our software is open source and hosted at: github.com/ourbigbook/ourbigbook
Further documentation can be found at: docs.ourbigbook.com
Feel free to reach our to us for any help or suggestions: docs.ourbigbook.com/#contact