is nido; and are arachno. The initial hydride removes an acidic bridging hydrogen as a proton, releasing and retaining the potassium counterion. Addition of one unit expands the boron framework; final protonation supplies the neutral hexaborane and KCl. These assignments conserve all the atoms in the displayed sequence, without inserting an unshown dehydrogenation step.
For , take one terminal B–H bond per vertex and remove its electrons from the valence total. The skeletal electron count is . ThusWade's rules assign , and pairs to closo, nido and arachno frameworks respectively. A derives from a six-vertex closo octahedron by removal of one vertex, giving a square-pyramidal boron skeleton. B and C have six-vertex open frameworks formally derived from an eight-vertex closo polyhedron by removing two vertices. Their additional hydrogens are distributed over bridging and other open-face positions; counting every hydrogen as an independent terminal B–H vertex would give the wrong classification.
The arachno assignment of has specific theoretical and NMR support. It should not be replaced by a permanently localized, unrearranged picture: the corresponding symmetric adduct participates in fluxional rearrangement rather than being the lowest-energy structure.[ref]
The Structure of arachno-B6H11-, at -25 degrees C in (CD3)2O, Is Resolved via the ab Initio IGLO-GIAO NMR Procedure by Matthias Hofmann and others. 2000, abstract: arachno minimum, bridging-hydrogen removal from B6H12 and alternative-adduct comparison
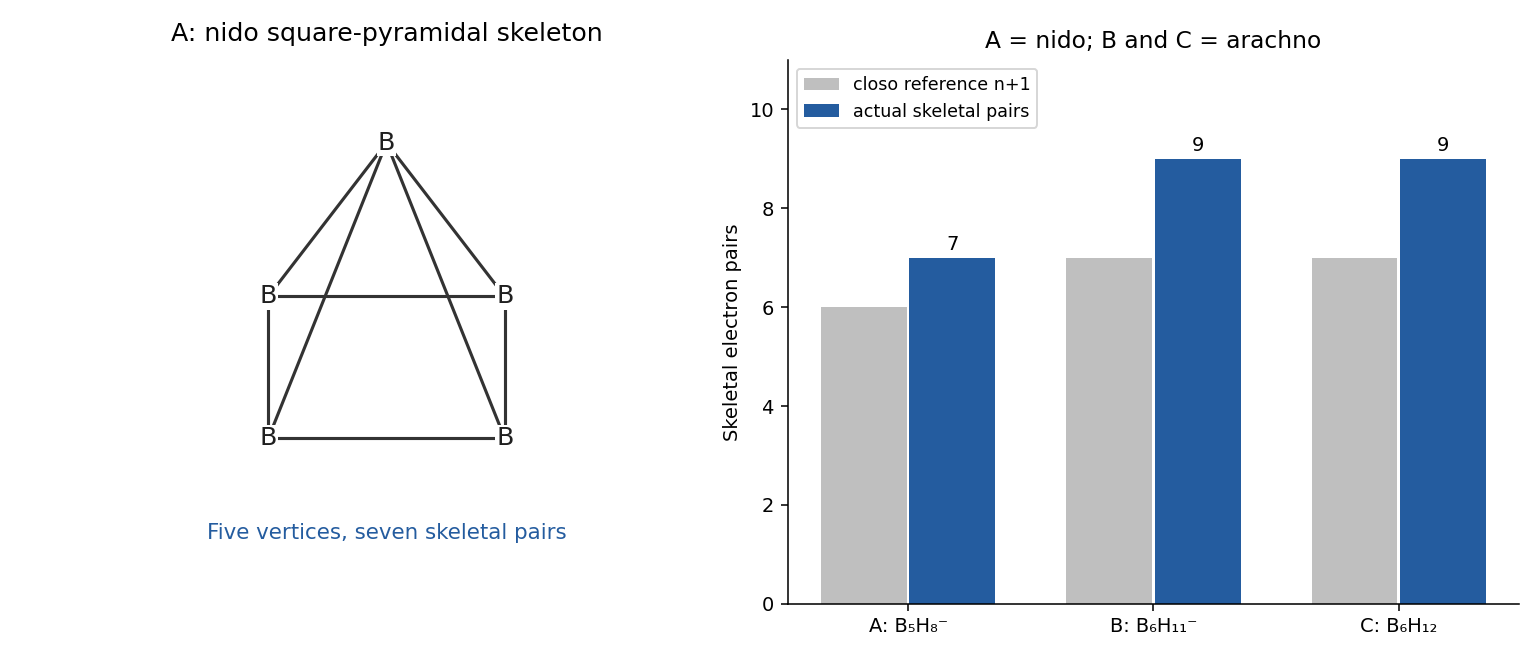

C, the neutral arachno , is the most plausible proton donor among A, B and C. Loss of an open-framework bridging proton produces the experimentally accessible, charge-delocalized conjugate base . In contrast, deprotonating A or B would build a dianion and incurs additional electrostatic cost. The neutral, open hydrogen-rich cluster therefore has a more favourable route to a monoanionic conjugate base. This is a qualitative acidity prediction for the listed species, not a numerical solvent-independent or a claim that all B–H hydrogens are equally acidic.
Articles by others on the same topic
There are currently no matching articles.