Topics (384k) Articles (398k) Users (410) Discussions (242) Comments (383) Files (13k) New article
Compactifying M-theory on a circle gives type IIA superstring theory. The circle radius sets its coupling. Multiplying M2-brane and M5-brane tensions by the circle circumference gives the fundamental string and D4-brane tensions, while unwrapped objects give D2-branes and NS5-branes. Momentum and a Kaluza-Klein monopole supply D0-brane and D6-brane charges. The circle dictionary and worldvolume reductions are developed in Four Lectures on M-theory.
M-theory on a two-torus and type IIB superstring theory on a circle describe the same nine-dimensional physics. Torus shape supplies the axion-dilaton; torus area supplies the circle-radius modulus after matching metrics. An M2-brane on a one-cycle gives a (p,q) string; an M5-brane on the whole torus gives a D3-brane. Matching brane charges and tensions establishes the dictionary in The Power of M Theory.
M-theory on a K3 surface and the heterotic string on a three-torus have matching seven-dimensional moduli and charge lattices. The K3 intersection lattice supplies twenty-two vector charges; an M5-brane wrapped on K3 becomes the heterotic fundamental string. The strong-coupling interpretation and low-energy matching are derived in section 4.7 of String Theory Dynamics in Various Dimensions.
Cytokinesis partitions the cytoplasm. Without cytokinesis, two cell nuclei can share one biological cell. [ref]
Cytokinesis makes physically separate daughter biological cells by partitioning their cytoplasm and completing their cell membrane boundaries. Mitosis divides nuclear material. These processes can overlap during M phase, but completion of one does not imply completion of the other.[ref]
The Cell Cycle. Biology 2e by Mary Ann Clark and others; §10.2, The Mitotic Phase and Cytokinesis: nuclear division versus physical daughter-cell separation
For an original compartment-counting example, consider a hypothetical diploid biological cell after two daughter cell nuclei have formed. Let be the number of chromosomes in one haploid set, and let be that set's unreplicated nuclear DNA amount, as in cell-cycle DNA content. Assume faithful mitosis, no nuclear DNA replication during the partition, and no loss of nuclear DNA; exclude mitochondrion DNA.
| Counting boundary | Before cytokinesis | After cytokinesis |
|---|---|---|
| Biological cells | 1 | 2 |
| Cell nuclei in each biological cell | 2 | 1 |
| Each cell nucleus | chromosomes, | chromosomes, |
| Nuclear DNA per biological cell | ||
| Nuclear DNA across all descendants |
The check is to follow the two existing cell nuclei: initially one boundary encloses both; finally each daughter boundary encloses one. The total remains two cell nuclei, twenty chromosomes and of nuclear DNA. Thus the amount per biological cell halves because the counting boundary changes, without any new DNA replication or change of nuclear ploidy. Doubling the number of biological cells need not double their combined material.
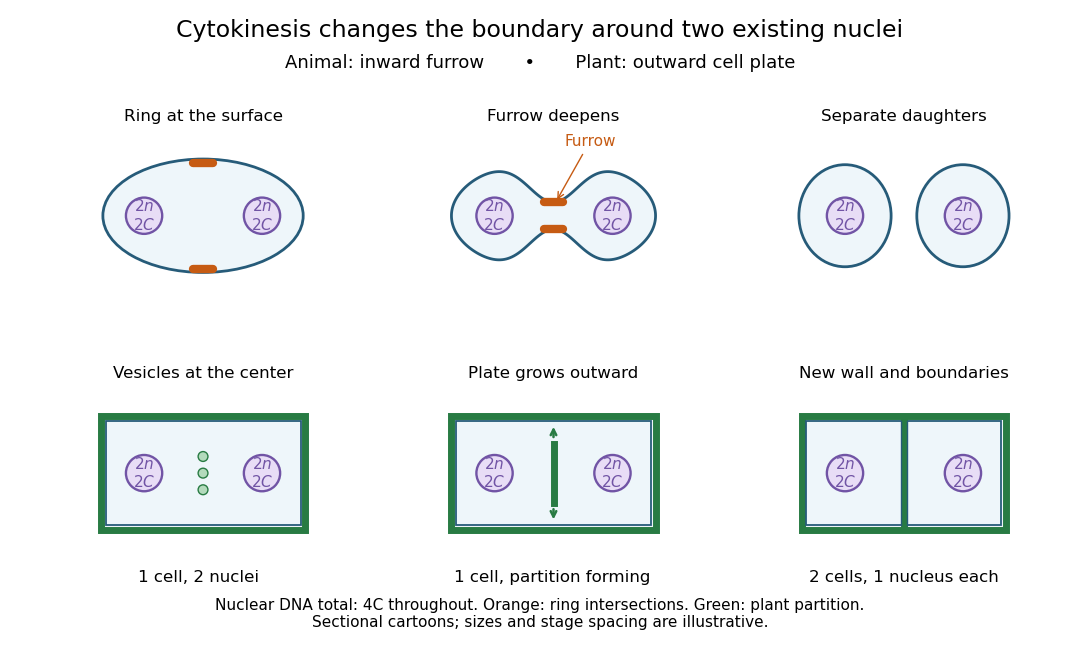
Coordinating chromosome segregation with cytoplasm partition lets descendants inherit nuclear information inside separate working compartments. Equal nuclear DNA allocations do not require equal daughter sizes or equal allocations of every organelle. The geometry of cytokinesis connects an internal allocation to the creation of two independently bounded biological cells.
Mitosis allocates copied chromosomes to daughter cell nuclei. The spindle apparatus aligns sister chromatids before separation in anaphase.
The copying has already occurred during S phase, before mitosis. Nuclear chromosome segregation and cytokinesis, the partition of the cytoplasm, are distinct processes: two daughter cell nuclei can form inside one undivided biological cell.[ref]
The Cell Cycle. Biology 2e by Mary Ann Clark and others; §10.2, Interphase and The Mitotic Phase; Figure 10.5: replication precedes nuclear division, which can occur without cytokinesis
The original cartoon follows a hypothetical diploid animal biological cell with . Its two homologous chromosome pairs are and ; upper- and lower-case letters identify homologues, not dominant and recessive alleles. In prophase and metaphase, each replicated chromosome contains two sister chromatids: four replicated chromosomes contain eight chromatids, rather than eight replicated chromosomes. The X shape depicts two associated copies, not the shape of every chromosome throughout the cell cycle.
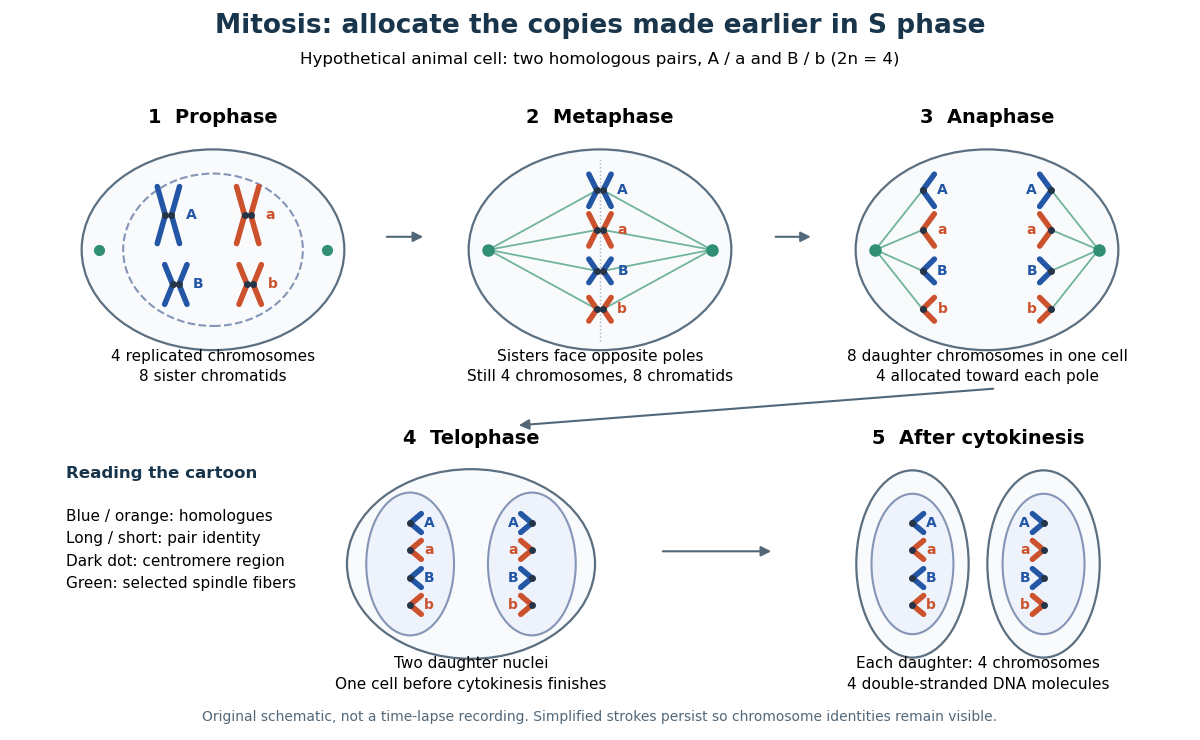
This open mitosis cartoon shows nuclear envelope breakdown and reassembly. Closed mitosis in some yeasts retains the nuclear envelope while daughter chromosomes separate inside it; the cartoon is therefore not a universal cellular architecture.[ref]
The Cell: A Molecular Approach, 2nd edition by Geoffrey M. Cooper. Chapter 8, The Nucleus during Mitosis, Dissolution of the Nuclear Envelope; Figures 8.29–8.30: open and closed mitosis
On a compact positively invariant set where , every trajectory approaches the largest invariant subset of .
For and , on either half-plane the Lyapunov function is nonnegative, has compact sublevel sets contained in that half-plane, and satisfies . The only invariant points of are and . The invariance argument therefore makes each half-plane converge to its corresponding stable focus. The stable set of the saddle at is exactly the line .
A Lyapunov functional assigns a scalar to the entire state of an evolution equation and is monotone along its trajectories. For a gradient flow , the identity follows from the variational chain rule, with boundary terms removed by periodicity or decay. A spatial density is not itself a Lyapunov functional unless all remaining coordinates are integrated or averaged.
For an open dust-only Friedmann-Lemaître-Robertson-Walker metric with zero cosmological constant and , . The present radial cosmological proper distance is , and the areal radial coordinate satisfies . Integrating with gives the displayed relation. It has near the observer and as . The luminosity distance is , not the radial cosmological proper distance.
In an Einstein-de Sitter universe normalized by , the Friedmann equation gives . Integrating the radial null geodesic gives . The luminosity distance is , yielding the displayed expression. Near the observer it is ; the limiting radial comoving distance is finite even though the luminosity distance diverges.
Spectral luminosity is energy radiated per unit time per unit frequency. Its frequency integral is the total luminosity. For an isotropic source at small distance , neglecting attenuation and cosmological effects, the spectral flux density is .
The luminosity per unit spatial volume. For a spherical source, its enclosed luminosity is , and its projected surface brightness is .
Fixed-quota harvesting of Lotka-Volterra populations by  Codex 0 Created 2026-10-14 Updated 2026-11-05
In logarithmic prey/predator coordinates, the Lotka-Volterra predator-prey model has divergence zero. Removing a fixed prey quota changes to and expands logarithmic area by . Thus a periodic annually harvested orbit has an expanding return map determinant and cannot be asymptotically stable. A continuous-quota approximation gives a coexistence equilibrium with positive Jacobian matrix trace , unlike proportional harvesting, which only changes the prey growth parameter in this idealized model.
An annual pulse-breeding predator-prey model combines continuous predation and mortality between short reproduction episodes with an annual difference equation. If surviving predators produce offspring in proportion to prey surviving the year, retained adults give the displayed map. Here combines prey reproduction and natural survival, is predator survival, and integrates predation over declining predator abundance. The positive annual equilibrium is , for and .
The velocity-addition formula translates a particle's velocity between two specified inertial frames. Let move at signed velocity along the -axis of , with parallel axes and , where is the speed of light. Define and for the same particle's world line, using position and time measured within the corresponding inertial frame. With Lorentz factor , the forward Lorentz boost gives
For collinear motion, write and . The inverse velocity-addition formula isThis is the composition of the particle's velocity in and that frame's velocity relative to . The velocities must belong to this same chain of reference frames, with directions specified. Two arbitrary quoted speeds cannot be inserted blindly. Each velocity measurement uses distances and clocks in a single inertial frame, with Einstein synchronisation for separated clocks.
For example, let and let the particle travel at in . Its velocity in isThe Galilean transformation would instead give , which fails here. For light moving along the positive axis, gives ; similarly gives . Negative directions also work for massive particles: at , gives , while gives . Thus “addition” means composition of signed velocities, rather than addition of their magnitudes.
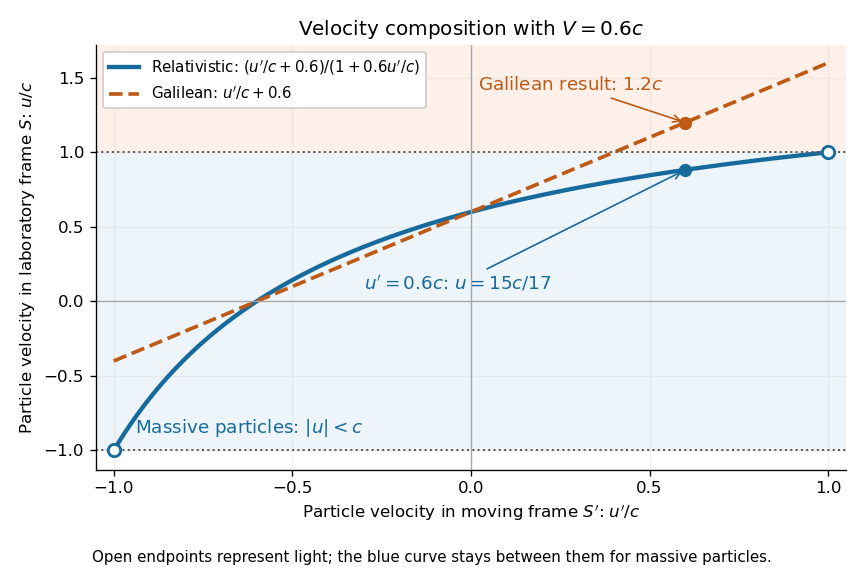
A short derivation differentiates the Lorentz transformation: and . Dividing these differentials gives the longitudinal velocity-addition formula. The transverse formulas use and , but the same transformed time denominator; omitting it would ignore the relativity of simultaneity. Replacing by gives the inverse. When both relative and particle velocities are small compared with the speed of light, the denominator is close to one and the nonrelativistic limit recovers the Galilean transformation.
The formula lets us compare particle motion in a moving apparatus and a laboratory without losing the invariant speed of light. Einstein's 1905 paper derives the coordinate change in §3 and the composition of velocities in §5, including the collinear formula, its light-speed case, and composition of parallel transformations. [ref]
https://www.fourmilab.ch/etexts/einstein/specrel/www/. Albert Einstein, On the Electrodynamics of Moving Bodies (1905), §§3 and 5; English translation by W. Perrett and G. B. Jeffery, electronic edition by John Walker
. The rapidity parametrization makes the collinear composition particularly simple.An orthonormal coframe in spacetime can be rotated by a position-dependent Lorentz matrix without changing the spacetime metric tensor. Its spin connection transforms as . A spinor field transforms through a chosen spin lift , not through the vector matrix . With , an infinitesimal parameter gives , where . Consistent global transition lifts require a spin structure; a spatial rotation lifts to minus the identity on spinors.
Lithium-7 has three protons and four neutrons. In Big Bang nucleosynthesis it can form directly or through beryllium-7, which later undergoes electron capture. Competition between direct lithium production, lithium destruction and beryllium production produces a valley in the primordial lithium abundance versus baryon-to-photon ratio. Its measured stellar surface abundance need not equal its birth abundance because stellar transport and nuclear burning can remove lithium.
A physiologist who developed the concept of homeostasis: interacting physiological processes maintain relatively stable internal conditions despite disturbances. In his account, stability is an actively maintained outcome rather than absence of ongoing change.[ref]
Homeostasis (excerpt from The Wisdom of the Body). 1932, opening discussion of resistance to changes

Portrait of Walter Bradford Cannon
. Wellcome Library, London / Wellcome Collection. CC BY 4.0, via Wikimedia Commons. Source.A membrane leaflet is one of the two layers forming a lipid bilayer. In a phospholipid-based cell membrane, the hydrophilic regions face the adjacent water, and the hydrophobic regions face the interior shared by the two membrane leaflets.
Pinned article: Introduction to the OurBigBook Project
Welcome to the OurBigBook Project! Our goal is to create the perfect publishing platform for STEM subjects, and get university-level students to write the best free STEM tutorials ever.
Everyone is welcome to create an account and play with the site: ourbigbook.com/go/register. We belive that students themselves can write amazing tutorials, but teachers are welcome too. You can write about anything you want, it doesn't have to be STEM or even educational. Silly test content is very welcome and you won't be penalized in any way. Just keep it legal!
Intro to OurBigBook
. Source. We have two killer features:
- topics: topics group articles by different users with the same title, e.g. here is the topic for the "Fundamental Theorem of Calculus" ourbigbook.com/go/topic/fundamental-theorem-of-calculusArticles of different users are sorted by upvote within each article page. This feature is a bit like:
- a Wikipedia where each user can have their own version of each article
- a Q&A website like Stack Overflow, where multiple people can give their views on a given topic, and the best ones are sorted by upvote. Except you don't need to wait for someone to ask first, and any topic goes, no matter how narrow or broad
This feature makes it possible for readers to find better explanations of any topic created by other writers. And it allows writers to create an explanation in a place that readers might actually find it.
Figure 1. Screenshot of the "Derivative" topic page. View it live at: ourbigbook.com/go/topic/derivativeVideo 2. OurBigBook Web topics demo. Source. - local editing: you can store all your personal knowledge base content locally in a plaintext markup format that can be edited locally and published either:This way you can be sure that even if OurBigBook.com were to go down one day (which we have no plans to do as it is quite cheap to host!), your content will still be perfectly readable as a static site.
- to OurBigBook.com to get awesome multi-user features like topics and likes
- as HTML files to a static website, which you can host yourself for free on many external providers like GitHub Pages, and remain in full control

Figure 2. You can publish local OurBigBook lightweight markup files to either OurBigBook.com or as a static website.
Figure 3. Visual Studio Code extension installation.
Figure 5. . You can also edit articles on the Web editor without installing anything locally. Video 3. Edit locally and publish demo. Source. This shows editing OurBigBook Markup and publishing it using the Visual Studio Code extension. 
- Infinitely deep tables of contents:




All our software is open source and hosted at: github.com/ourbigbook/ourbigbook
Further documentation can be found at: docs.ourbigbook.com
Feel free to reach our to us for any help or suggestions: docs.ourbigbook.com/#contact