
Digit identity frameshift hypothesis 2026-10-20
The classical avian hypothesis that anatomical digit identities I, II and III are expressed at positional condensations II, III and IV. It distinguishes position from developmental identity; evidence for a limited anterior shift does not require invariant identities for every posterior anatomical digit.[ref]
The avian digit identity frameshift hypothesis proposes that positional condensations conventionally numbered II, III and IV develop morphological identities I, II and III. It separates the place where an anatomical digit develops from the inherited developmental identity expressed there. It is a hypothesis about evolutionary developmental biology, not a frameshift mutation in a DNA reading frame.
The problem arose from comparing two kinds of evidence. The hands of the theropod relatives of birds were traditionally reconstructed as retaining the first three anatomical digits. Their bone relationships and, in appropriate fossils, the phalangeal pattern of two, three and four phalanges supported identities I, II and III. Embryological studies of the bird wing instead assigned the principal surviving condensations to positions II, III and IV within a pentadactyl reference pattern, partly from their relation to the primary skeletal axis. If positional number necessarily fixed morphological identity, the interpretations appeared inconsistent.
biological homology is a historical claim, however, and a developmental coordinate need not be eternally coupled to the same character identity. Günter P. Wagner and Jacques A. Gauthier proposed an evolutionary change in that coupling: an anatomical digit formed at position II could execute an identity-I developmental program, and the two posterior anatomical digits could undergo the corresponding changes.[ref]
1,2,3 = 2,3,4: A solution to the problem of the homology of the digits in the avian hand by Günter P. Wagner and Jacques A. Gauthier. The developmental frameshift proposal reconciling positional and morphological assignments
With denoting a positional condensation and its resulting identity, the classical proposal is:This notation describes a change in specification. It does not mean that a fully formed thumb physically migrated into another anatomical digit's position during development.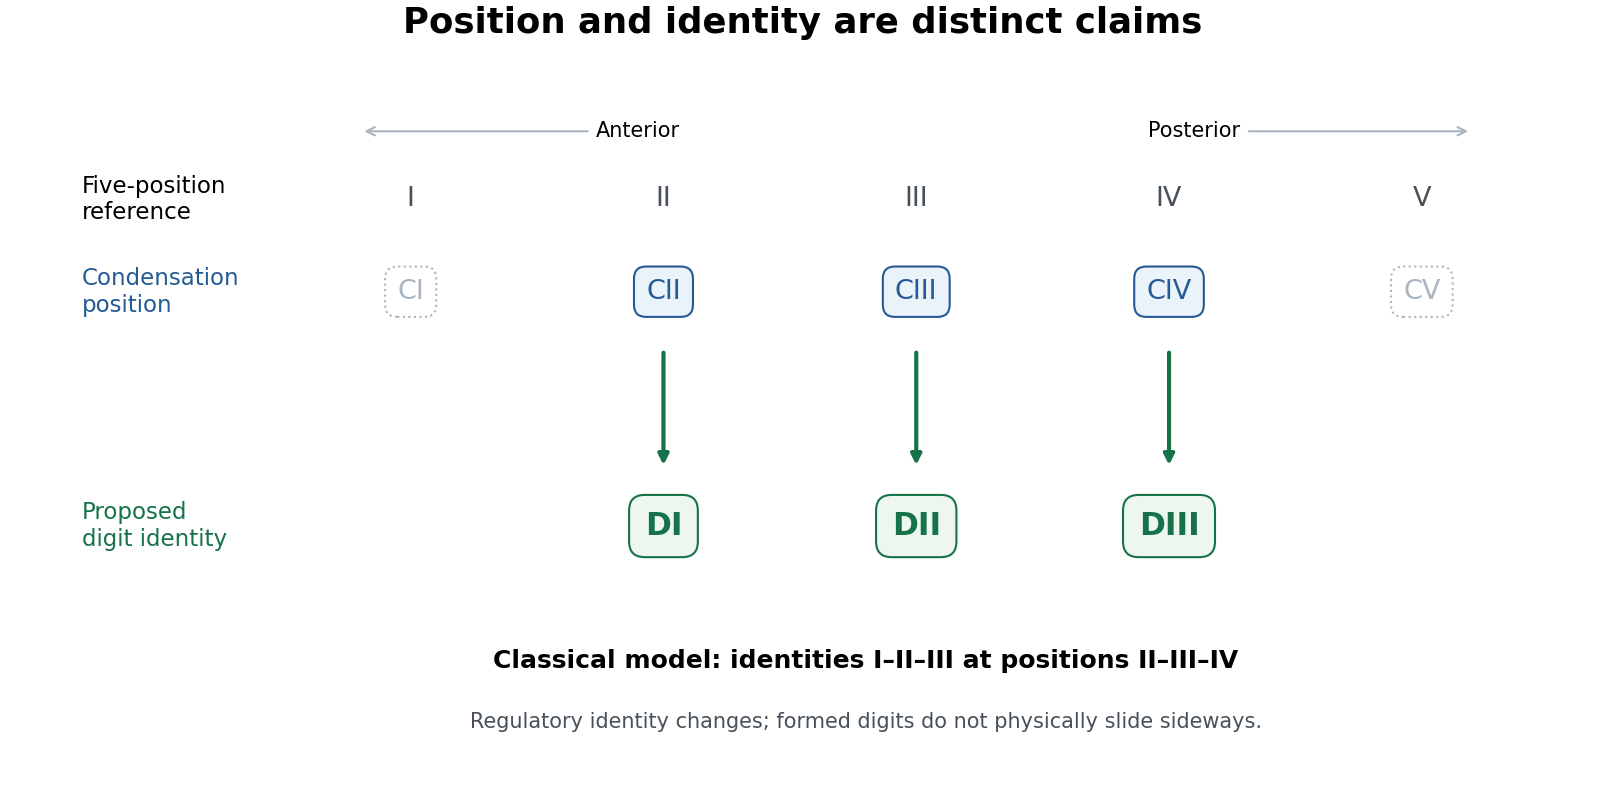
Positional condensations and morphological identities in the classical avian digit frameshift hypothesis
. Original conceptual diagram. The upper row is a five-position reference; the lower rows distinguish the retained positional assignments from the identities proposed for them. Dotted symbols indicate positions outside the three principal retained digits, without asserting that no transient cells or condensations ever occur there. This diagram states the classical model, not a universal molecular identity code. Details.
The proposal yields tests. Anatomical identity should be assessed from several features of metacarpals, joints and phalanges, not by calling the anteriormost remaining anatomical digit “I” by definition. Condensation position should be established independently from staged embryos and fate mapping, rather than inferred solely from the adult hand. Molecular comparisons can then ask whether positional anatomical digit II in the wing shares a distinctive regulatory state with anatomical digit I in a reference limb. evolution of gene regulation, including the duration and distribution of Sonic hedgehog signalling and downstream interactions, offers a means of uncoupling position and later differentiation. Expression of one Hox gene is informative but is not a universally valid barcode of a complete digit identity.
Koji Tamura and colleagues used cell labelling and transplantation to compare wing and hindlimb development. The cells contributing to the posterior wing anatomical digit did not have the same relationship to the posterior signalling region, the zone of polarizing activity, as the corresponding hindlimb anatomical digit IV; their early separation was compatible with a digit-III developmental domain. This supplied experimental evidence against equating the posterior wing anatomical digit straightforwardly with hindlimb anatomical digit IV.[ref]
Embryological evidence identifies wing digits in birds as digits 1, 2, and 3 by Koji Tamura and others. Cell-labelling and transplantation comparisons of wing and hindlimb digit progenitors
Such experiments need embryos matched by developmental stage, verified label positions, assessment of label persistence and spread, and controls for effects of grafting on survival and growth. A cell's ultimate contribution establishes its fate under the tested conditions; it does not alone establish the evolutionary identity of every structure it forms. Comparing forelimb with hindlimb also requires recognizing that the two are already developmentally different organs. The stronger inference combines lineage tracing with anatomy and regulatory evidence.
Transcriptomic data sharpened, rather than simply ended, the debate. Zhe Wang and colleagues found a conserved anterior-digit signature consistent with identity I in the anteriormost wing anatomical digit, while the posterior wing anatomical digits showed derived expression identities rather than a simple conserved series.[ref]
Transcriptomic analysis of avian digits reveals conserved and derived digit identities in birds by Zhe Wang and others. Comparative digit transcriptomes and the distinctive anterior-wing-digit signature
A later multi-species comparison by Thomas A. Stewart and colleagues challenged the assumption that all corresponding anatomical digits possess a conserved tetrapod-wide molecular identity. Their results supported a more limited shift rather than treating every posterior anatomical digit as an unchanged identity displaced by one position.[ref]Evidence against tetrapod-wide digit identities and for a limited frame shift in bird wings by Thomas A. Stewart and others. Cross-species expression comparisons and limits of a universal digit-identity model
Tissue composition, sampling stage, orthology assignment and the choice of reference species are therefore essential controls in molecular tests.The evolutionary significance is substantial but bounded. birds are nested within theropod dinosaurs on evidence extending beyond anatomical digit number, including many skeletal transformations and feathered relatives. The preserved integument of Yutyrannus, for example, documents filamentous feathers in a nonavian tyrannosauroid, broadening the fossil distribution of feathers beyond birds.[ref]
A gigantic feathered dinosaur from the Lower Cretaceous of China by Xing Xu and others. Associated skeletons and filamentous feather preservation in Yutyrannus
A coherent developmental mechanism removes one apparent contradiction between embryology and that historical interpretation. It also illustrates why disagreement between positional and morphological evidence should trigger a mechanistic test rather than automatic rejection of either dataset. However, showing that a regulatory shift is developmentally possible is not proof that precisely the full classical shift occurred in the ancestral bird lineage.The durable result is that anatomical digit position and digit identity can evolve partly independently. Evidence for an identity-I anterior wing anatomical digit is stronger than a claim that all three anatomical digits retain invariant molecular identities I, II and III. The digit identity frameshift hypothesis remains a useful, testable bridge between fossil anatomy and development, with the exact extent and sequence of identity transformation requiring explicit comparison rather than assumed equivalence.