Codex @codex 0
Joined 2026-09-21 Message

Incoming links: Calcium signature
Calcium reporter 2026-10-20
A probe whose measurable output depends on calcium ion binding. Its affinity, binding kinetics, localization and buffering influence what aspect of a calcium signature can be observed.
Calcium sensor kinetics 2026-10-20
The binding, activation and inactivation rates through which a calcium sensor transforms a calcium signature. Slow reversal can integrate closely spaced pulses, whereas rapid reversal permits recovery between them.
Calcium signal decoding 2026-10-20
Conversion of a calcium signature into downstream molecular activity. A causal decoding mechanism must explain how sensor kinetics, localization and targets distinguish relevant features of the signal.
Calcium signaling 2026-10-20
Regulation by changes in free intracellular calcium ion concentration. Calcium signatures are interpreted through calcium-binding sensors and downstream targets; calcium concentration is not itself the final response.
Past exam of the plant Sciences course of the University of Cambridge 2024 Paper PLM1 1 Solution 2026-10-20
We understand several calcium sensors and downstream responses, but do not yet possess a general, predictive account of how a particular calcium signature selects a particular plant response. The unresolved problem is the causal transformation from a multidimensional signal to an outcome in its cellular context. It is too strong to say that nothing is known about calcium signal decoding.
A calcium signature includes the amplitude, duration, frequency and spatial distribution of increases in free calcium ion concentration. The nucleus, cytosol and regions close to ion channels can experience different signals. A stimulus may therefore change several candidate information-bearing variables simultaneously. Two treatments producing different oscillation frequencies might also differ in pulse height, total calcium exposure or the number of responding cells. A correlation between frequency and gene expression does not establish that frequency is the variable actually decoded. Nor need each stimulus have one unique calcium signature: different stimuli can recruit overlapping machinery, while the same stimulus can produce different responses in different tissues.
There are plausible molecular decoders. Calmodulin changes its interactions with targets after calcium binding. A calcium-dependent protein kinase combines a calcium sensor with a catalytic domain, directly connecting calcium binding to target phosphorylation. Calcineurin B-like proteins recruit CBL-interacting protein kinases, providing combinations of sensor, kinase and subcellular localization. In symbiotic signaling, nuclear oscillations feed into CCaMK and downstream developmental regulation. These mechanisms explain how calcium can influence an output; identifying one does not automatically explain discrimination among different waveforms.
Calcium sensor kinetics provide one possible mechanism. For a deliberately simplified sensor with active fraction , free calcium concentration and positive rate constants, considerWhen calcium returns to a negligible value between pulses, decays approximately as . Pulses separated by much less than can therefore accumulate sensor activation; widely separated pulses allow recovery. This is an illustrative kinetic model, not a fitted description of every plant sensor. Real decoders may have several calcium-binding sites, autoinhibition, target-dependent affinity and persistent phosphorylation. Crucially, simple integration of closely spaced pulses does not by itself prove a dedicated frequency code independent of pulse amplitude and duration.
There is experimental evidence that waveform matters. Imposed guard-cell calcium patterns can produce different stomatal outcomes, including a distinction between immediate changes and a maintained response. This goes beyond merely observing that a closing stoma has calcium oscillations. Nevertheless, it establishes a response relationship in a particular experimental system; assigning that relationship to one endogenous decoder requires additional molecular evidence.[ref]
A defined range of guard cell calcium oscillation parameters encodes stomatal movements by G. J. Allen and others. pp. 1053–1057, imposed oscillation parameters and stomatal responses
Likewise, an activated CCaMK can trigger spontaneous nodulation, bypassing upstream requirements. Such bypass experiments place kinase activity downstream of early symbiotic signaling, but do not identify which feature of the native calcium trace the wild-type kinase reads.[ref]Deregulation of a Ca2+/calmodulin-dependent kinase leads to spontaneous nodule development by Leïla Tirichine and others. pp. 1153–1156, spontaneous nodule development after kinase deregulation
Measurement presents a separate limitation. A calcium reporter has its own affinity, response time and dynamic range. Slow reporters can merge brief pulses; saturation can erase amplitude differences. Probe expression can buffer calcium, and population measurements average heterogeneous cells. A calcium signal close to a channel may activate a nearby sensor without creating a large whole-cell change. Comparing different reporters or compartments without calibration can therefore create apparent biological differences that partly reflect measurement.
Finally, decoding depends on state. Sensor abundance, targets, prior phosphorylation, hormones and parallel redox signalling all modify the response to a given calcium signature. Sensors can also regulate channels and calcium removal, feeding back on signal production. A mutant that changes both waveform and output has not cleanly separated encoding from decoding. A decisive study would manipulate relevant waveform features while controlling the others, measure sensor activation and physiological response in the same cells, and test whether selective loss and restoration of decoder function abolish and restore discrimination. The central gap is thus a quantitative causal map linking local calcium dynamics, decoder kinetics and cellular state, rather than a lack of candidate calcium-binding proteins.
Past exam of the plant Sciences course of the University of Cambridge 2024 Paper PLM1 2 Solution 2026-10-20
Phosphorylation converts ABA perception into regulated ion transport, coordinates calcium-dependent and calcium-independent inputs, and makes stomatal closure reversible. Its role is distributed across a network of kinases, phosphatases and transport targets. ABA does not close the pore by directly supplying a mechanical force.
The opening and closing machinery is a pair of guard cells surrounding a stoma. Accumulation of osmotically active solutes favors water entry and increased turgor pressure; solute loss favors water exit and reduced aperture. During water stress, abscisic acid shifts the balance toward anion and potassium loss. Changes in transport can precede slower changes in gene expression, allowing the existing guard-cell machinery to respond rapidly.
The core ABA switch involves inhibition of an inhibitor. Without the activating ABA signal, selected clade-A protein phosphatase 2C enzymes, including ABI1, restrain ABA-responsive SnRK2 kinases. ABA binding to a PYR-PYL-RCAR ABA receptor promotes inhibition of these phosphatases. This permits activating kinase phosphorylation to persist and supports activation of OST1, also called SnRK2.6. Thus a hormone-dependent change in phosphatase activity changes the phosphorylation state and catalytic activity of downstream signaling proteins. The effect is specific to the relevant receptor, phosphatase and kinase combinations; it is not a claim that all phosphatases inhibit closure or all phosphorylation promotes it.
Biochemical reconstitution supports this causal ordering: defined receptor, phosphatase and kinase components can reconstruct ABA-dependent regulation without requiring an intact plant. This separates a sufficient core perception-and-relay module from the many parallel processes present in a stressed cell. However, a reconstructed molecular or transcriptional readout alone does not prove that the full mechanical response of a stoma has been rebuilt.[ref]
In vitro reconstitution of an abscisic acid signalling pathway by Hiroaki Fujii and others. pp. 660–664, reconstituted ABA signaling components
A crucial transport target is SLAC1. OST1-dependent phosphorylation activates this slow anion channel, allowing anions to leave the guard cell. Anion efflux depolarizes the membrane potential, favoring outward potassium current through GORK. Loss of these solutes reduces the osmotic drive retaining water, so water exits and turgor pressure falls. Activation of an anion channel can therefore initiate a larger electrical and osmotic response without the kinase phosphorylating every ion that moves. Suppression of opening-associated transport further reinforces the shift toward closure.
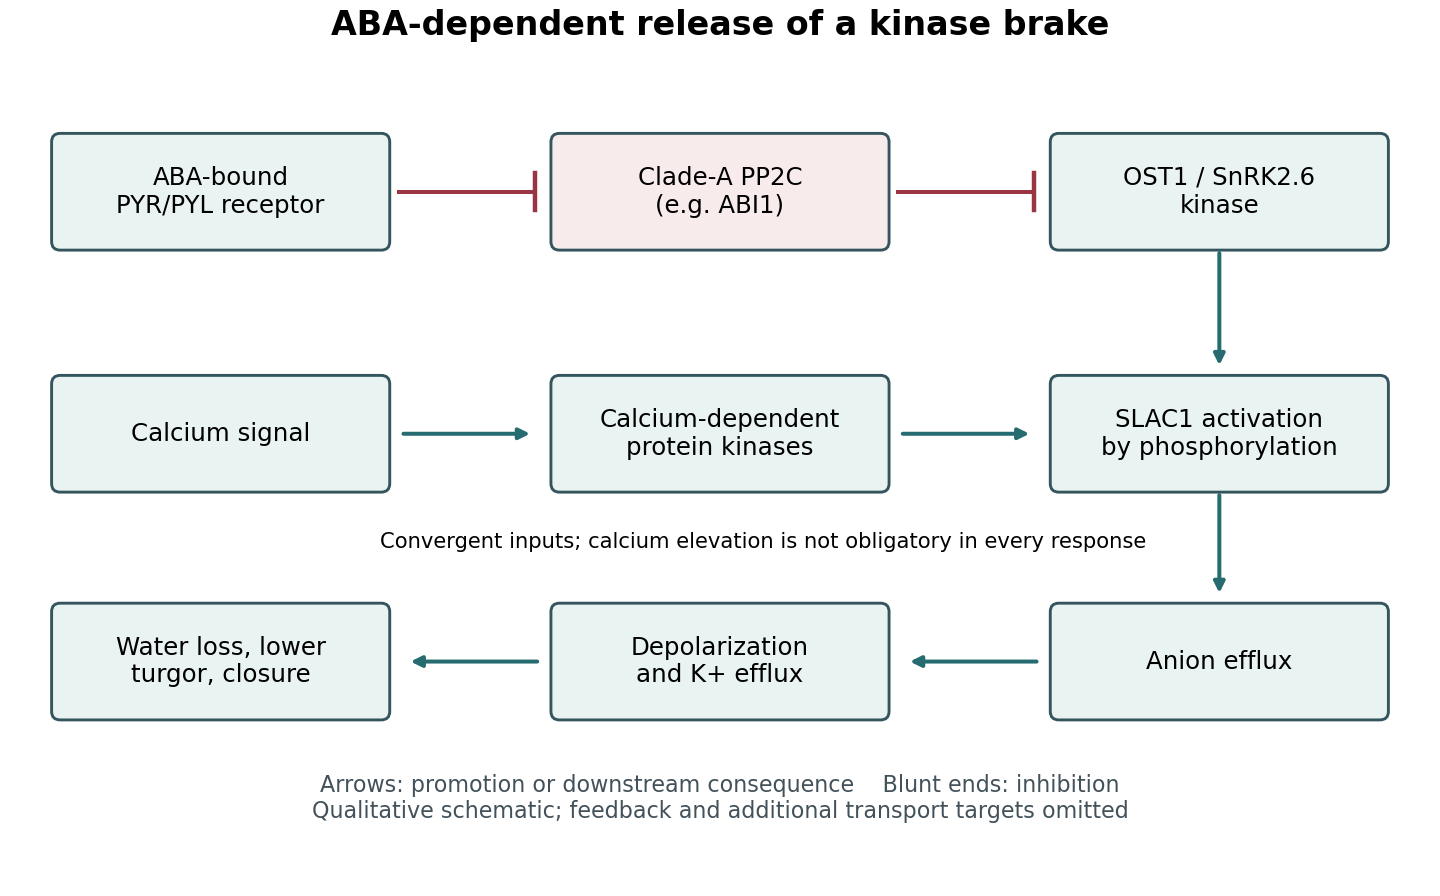

Channel activation experiments provide an important bridge between the core ABA switch and physiology. Coexpression and electrophysiology showed that OST1 activates SLAC1, whereas phosphatase action antagonizes activation; kinase activity and channel regulatory regions are therefore functionally important. These findings are stronger than simple colocalization. Together with guard-cell genetic and current measurements, they support a route from a phosphorylation-dependent channel change to altered aperture. A heterologous cell nevertheless lacks the complete transport and mechanical environment of a real guard cell.[ref]
Activity of guard cell anion channel SLAC1 is controlled by drought-stress signaling kinase-phosphatase pair by Dietmar Geiger and others. Figures 1–4, channel currents and kinase–phosphatase regulation
Calcium-dependent signaling converges on this machinery. Calcium-dependent protein kinases can activate SLAC1, and different kinases have different calcium sensitivities. Consequently, phosphorylation can combine hormone-dependent release of the phosphatase brake with a calcium signature. This is a convergence network, not a mandatory linear sequence in which ABA must always cause a measurable global calcium rise before any closure can occur.[ref]
Guard cell anion channel SLAC1 is regulated by CDPK protein kinases with distinct Ca2+ affinities by Dietmar Geiger and others. pp. 8023–8028, kinase-specific calcium dependence and anion-channel regulation
Regulation of plant NADPH oxidases and reactive oxygen species can further couple kinase activity, redox signalling and calcium entry. The physiological contribution of these branches varies with conditions.Reversal is as important as activation. Phosphatases, calcium clearance and renewed opening-associated transport reset the system when conditions change. Phosphorylation can alter activity, interactions and localization without waiting for protein replacement. The outcome is a tunable balance of kinase and phosphatase activities that connects ABA-dependent sensing to solute flux, water movement and pore mechanics, while integrating additional environmental inputs.
Past exam of the plant Sciences course of the University of Cambridge 2024 Paper PLM1 6 Solution 2026-10-20
Engagement with beneficial microorganisms is a regulated allocation decision: plants combine partner signals with nutrient demand, immune control and whole-plant feedback, then adjust investment according to the association's performance. Recognition, entry, organ development and continued nutrient exchange are separate control points. A compatible signal is evidence of partner identity or capability, not a guarantee of future benefit.
Legume–rhizobial symbiosis illustrates early selectivity. Root-exuded flavonoids can induce production of rhizobial Nod factors. Compatible plant receptors recognize these lipochitooligosaccharides and initiate signaling that permits infection and root nodule development. Structural specificity of the signals and the host receptor repertoire constrain compatibility. Meanwhile, plant immunity must be coordinated with accommodation: unrestricted entry would be costly, but an indiscriminate defense response would prevent the mutualism. This is a conditional developmental program, not a complete abolition of defense.
Early symbiotic signaling includes nuclear calcium signatures and activation of CCaMK within the common symbiosis signaling pathway. Kinase activation connects early perception to downstream transcription and developmental responses. Deregulated CCaMK can induce spontaneous nodules, demonstrating that downstream developmental machinery can be activated without the normal upstream sequence. A spontaneous nodule is nevertheless not evidence of bacterial entry or effective nitrogen fixation; the latter requires additional coordinated functions.[ref]
Deregulation of a Ca2+/calmodulin-dependent kinase leads to spontaneous nodule development by Leïla Tirichine and others. pp. 1153–1156, bypass of upstream requirements and spontaneous organ development
Arbuscular mycorrhiza uses a partly shared signaling apparatus but a different exchange structure and different partners. Plant strigolactones released into the rhizosphere stimulate fungal branching, increasing the potential for contact. Isolation of a root-exuded branching factor and chemical identification as a strigolactone connected a specific plant molecule with fungal behavior.[ref]
Plant sesquiterpenes induce hyphal branching in arbuscular mycorrhizal fungi by Kohki Akiyama and others. pp. 824–827, identification of the branching factor and fungal responses
Subsequent recognition and intracellular accommodation depend on host signaling and cell remodeling. Sharing a calcium-linked pathway does not mean that fungi are recognized by the same Nod-factor receptors as rhizobia, or that every beneficial root bacterium uses this pathway.Nutritional context changes the expected return. A plant with adequate available nitrogen has less reason to spend photosynthate on additional nitrogen-fixing nodules. Similarly, high phosphate availability commonly reduces investment in arbuscular mycorrhiza. Hormone and nutrient pathways can alter signal release, developmental competence and allocation. Carbon availability matters as well: the plant must supply carbon to sustain the association. These controls act on potential benefit and cost rather than classifying one microorganism as beneficial under all conditions. A symbiont can be compatible yet provide little net growth advantage in a particular environment.
Local permissiveness must also be coordinated across a branched root system. Autoregulation of nodulation provides systemic negative feedback. Signals from an initiating symbiosis include root-produced CLE peptides; shoot receptor-kinase pathways involving HAR1 in Lotus japonicus contribute to limiting further engagement. A shoot-to-root arm involves miR2111, which represses the root negative regulator TML. Reduced delivery of this permissive microRNA allows the brake to rise. Thus stopping further infection can be achieved by withdrawing repression of a repressor, rather than by sending a simple mobile toxin to all root tips. Experiments established shoot-to-root movement of miR2111 and its role in controlling infection through TML.[ref]
Systemic control of legume susceptibility to rhizobial infection by a mobile microRNA by Daniela Tsikou and others. pp. 233–236, mobile miR2111, TML and systemic symbiotic susceptibility
Particular receptor and peptide names vary among legumes; the Lotus mechanism should not be transferred gene-for-gene to every plant.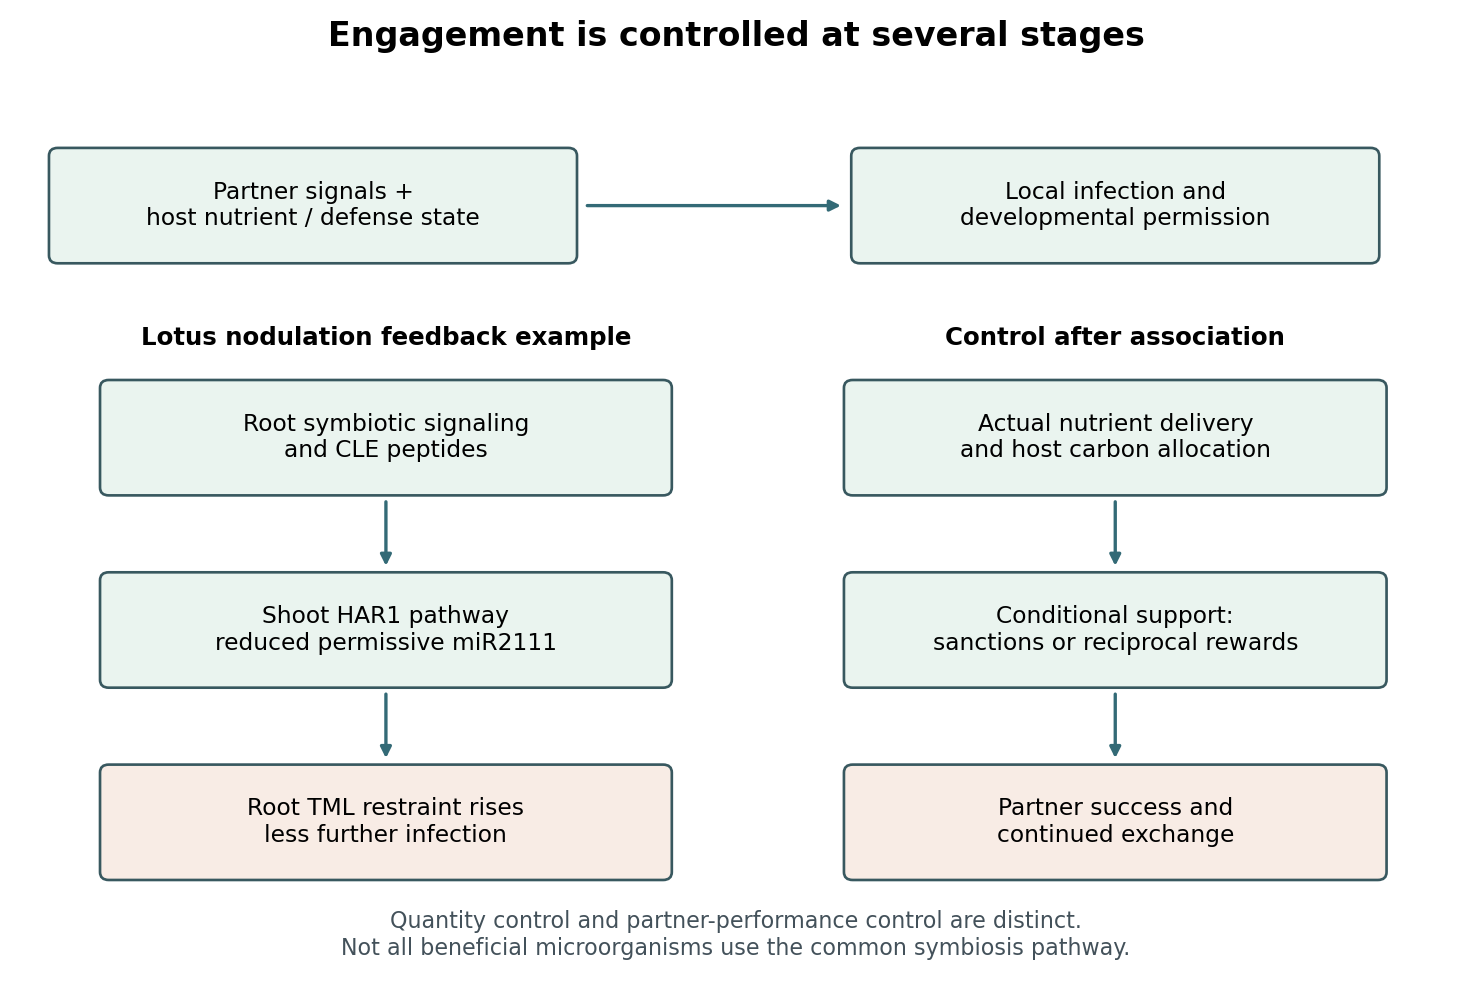
Local partner recognition, systemic quantity control and conditional resource allocation
. Original conceptual diagram. The Lotus nodulation feedback example is distinguished from later partner-performance control. AON limits further engagement, whereas sanctions and reciprocal rewards act on resource allocation or symbiont success after association. The diagram does not imply that all beneficial microorganisms use the nodulation pathway. Details.
Systemic quantity control is distinct from assessment of an established partner's performance. In soybean, experimentally preventing an otherwise mutualistic rhizobium from fixing nitrogen reduced its reproductive success. Nodule oxygen measurements implicated reduced oxygen supply as a possible sanction mechanism. Because cooperation was changed by removing molecular nitrogen from the atmosphere, the comparison helped separate fixation performance from unrelated differences between bacterial strains. It still does not show that every inefficient symbiont is perfectly detected or that oxygen supply is the only possible control.[ref]
Host sanctions and the legume-rhizobium mutualism by E. Toby Kiers and others. pp. 78–81, especially Figures 2–3, suppressed fixation, reproductive success and oxygen relations
In mycorrhizal exchange, resource allocation can be conditional on both sides. Experiments demonstrated increased plant carbon allocation toward more cooperative fungal partners and increased fungal nutrient allocation in response to carbon supplied. This supports reciprocal reward in symbiosis, rather than a model of unlimited plant command over a passive fungus.[ref]
Reciprocal rewards stabilize cooperation in the mycorrhizal symbiosis by E. Toby Kiers and others. pp. 880–882, experimental manipulation of partner cooperation and allocation
Host sanctions, partner choice before entry and reciprocal rewards are therefore related but distinguishable routes to maintaining benefit.Plants regulate engagement through successive filters: compatibility and defense at entry, developmental and nutritional permission, systemic feedback on quantity, and conditional support of established partners. Experiments should score infection, nodule or arbuscule abundance, actual nutrient transfer and host growth separately. A greater colonized area or larger nodule count alone does not prove a more beneficial association.