Both conflicts arise because family members value the same resource differently, but they concern different decisions. Sibling rivalry concerns allocation among offspring, whereas parent-offspring conflict concerns a parent's allocation relative to what an offspring would favour. Their consequences interact: offspring compete with one another inside a parental provisioning system that their own demands can also alter.
The basic mechanism is unequal genetic relatedness to the beneficiaries of an action. An offspring values its own additional survival or reproduction more strongly than an equal gain to a sibling. A parent, under a simple symmetric pedigree, is equally related to each of its offspring and can favour an allocation that maximizes their combined contribution. Neither statement implies that an offspring should demand everything: diverting resources from relatives can reduce its inclusive fitness. These differing interests underlie the original theory of parent-offspring conflict.[ref]
Parent-Offspring Conflict by Robert L. Trivers. 1974, theory of investment, sibling costs and the duration of care
Consider an explicit illustrative model. Let investment produce a direct offspring benefit and an opportunity cost measured in lost equivalent fitness contributions of other offspring. Assume a single parent, equal value of current and future offspring, no inbreeding, and relatedness between the focal offspring and those losing resources. After dropping a common parental relatedness factor, the parent's objective is , whereas the offspring's is . Interior optima therefore satisfyWith diminishing marginal benefits and , the offspring typically favours more investment. In particular, the range contains increments favoured by the offspring but opposed by the parent. For full siblings under the stated pedigree, ; for maternal half-siblings, . These values are not universal constants for all family structures, and parent survival, reproductive value and density dependence can alter the effective costs.
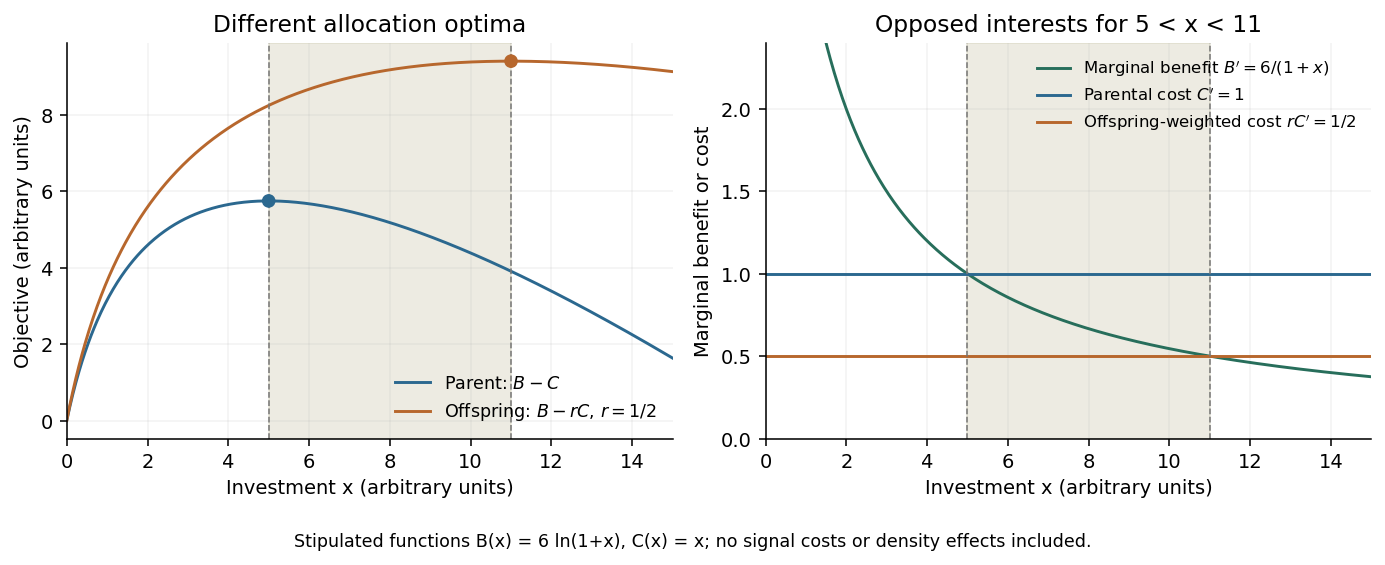
An original illustrative allocation model separates parental and offspring optima
. Chosen functions and give a parental optimum at and a full-sibling-weighted offspring optimum at . The shaded interval contains increments whose marginal benefit is below the parental opportunity cost but above the offspring-weighted cost. These are stipulated functions and arbitrary units, not empirical measurements. Details.
Sibling rivalry selects on relative access; parent-offspring conflict can also change the total supply. If one nestling obtains a larger fraction of a fixed food delivery, its sibling loses directly. Selection can favour size advantages, advantageous positions, earlier hatching or more effective solicitation. Severe asymmetries can permit siblicide or brood reduction. By contrast, a stronger demand directed at a parent can increase food delivery to the brood, potentially benefiting siblings too. The same begging behaviour can therefore redistribute a fixed supply and alter parental effort, with different consequences in each case.
A parent's preferred distribution need not be equal. A marginal food item may produce more surviving descendants when given to a smaller hungry chick, or to a larger chick that alone can survive a severe shortage. Parental allocation can consequently mitigate sibling asymmetry in one environment and reinforce it in another. Asynchronous hatching and brood-size adjustment are plausible parental means of structuring that contest; whether a particular asymmetry is an adaptation, a constraint or an offspring-driven outcome needs evidence. A parent's tolerance of brood reduction is not proof that every aggressive act serves parental interests.
Over evolutionary time, sibling rivalry can affect competitive morphology, growth schedules, solicitation, nest position and the survival distribution within broods. Parent-offspring conflict can affect the amount and duration of care, offspring demand, parental responsiveness, weaning schedules and the trade-off between current and future reproduction. Neither conflict predicts unlimited escalation. Energetic expenditure, injury, predation risk and losses to relatives can make competitive effort costly even when it obtains a larger resource share.
Information can produce compromise as well as waste. An offspring usually has private information about its hunger, while the parent integrates brood condition with its own prospects. In a costly-signalling model, offspring in greater need gain more from additional resources, so differing incentives can support informative solicitation at equilibrium. Such a result is conditional on the cost and benefit functions; it does not mean all begging is perfectly honest or that energetic expenditure alone establishes honesty.[ref]
Signalling of need by offspring to their parents by H. C. J. Godfray. 1991, primary signalling model and its assumptions
Signals can also be aimed at siblings. Experiments on barn owls found that nestlings reduced vocalization when a rival was hungrier, increased it after that rival was fed, and altered calling with experimental brood size. These calls occurred when parents were absent. They support sibling negotiation: assessing relative willingness to contest a future prey item can avert some unnecessary escalation. The experiment therefore cautions against treating every nestling call as a demand directed at the parent.[ref]
Barn owl (Tyto alba) siblings vocally negotiate resources by Alexandre Roulin and others. 2000, hunger and brood-size manipulations
A further consequence is coevolution among parental and offspring response rules. A demand phenotype expressed in young becomes part of the selective environment of provisioning adults, while parental allocation changes the returns to offspring competition. The same individual can experience both roles at different life stages, and genetic correlations between demand and care can constrain independent optimization. Thus observed care can be a compromise maintained by interacting strategies rather than the optimum of either party in isolation.
The comparison is consequently about overlapping arenas of selection. Sibling rivalry chiefly determines who obtains care, while parent-offspring conflict also determines how much care is supplied and when it ends. Both can generate competitive adaptations and costs, but both can also generate assessment, contingent responses and restraint. A strong empirical test must separate changes in total provisioning from redistribution, measure lifetime consequences rather than only immediate feeding success, and manipulate relatedness or information without simultaneously changing need.
Articles by others on the same topic
There are currently no matching articles.