cetaceans illustrate a sequence of inherited mammalian features, terrestrial specializations and subsequent aquatic transformations, followed by divergence in feeding and sensory anatomy. This is a branching phylogenetic tree, not a procession of named fossils that can all be identified as direct ancestors. Here Cetacea includes living whales, dolphins and porpoises; mammals means the crown group containing living monotremes and therians, whereas mammaliaforms also includes close extinct relatives outside that crown group. Dates below are approximate millions of years ago, abbreviated Ma.
The starting condition is a terrestrial, non-mammaliaform cynodont, itself a therapsid within Synapsida. Along the mammalian stem group, enlargement of the dentary and reduction of the other lower-jaw bones accompanied more differentiated teeth, increasingly precise dental occlusion and elaboration of a secondary palate. These changes belong to a feeding and respiratory complex: a larger tooth-bearing bone carries the mastication load, differentiated teeth process food, and a bony partition separates nasal and oral passages. They were acquired in a mosaic; neither a full modern mammalian jaw nor the aquatic body plan appeared at the initial divergence from other cynodonts.
Early mammaliaforms show how jaw support and hearing became reorganized. Morganucodon, around the Triassic–Jurassic transition and Early Jurassic, retained the old articular–quadrate jaw joint alongside a dentary–squamosal joint. In the mammalian condition the dentary–squamosal articulation supports the jaw, while the articular and quadrate correspond to the malleus and incus; the angular bone contributes to the ectotympanic. This is biological homology supported by comparative anatomy and biological development, not merely similarity in function. Hadrocodium, about 195 Ma, records further changes in jaw attachment and the braincase consistent with increased separation of mastication and hearing. Its tiny skull does not preserve an entire living-style ear apparatus; the reconstruction depends partly on bony attachment evidence. [ref]
The inherited mammalian package also includes diphyodonty, hair and lactation, although the latter two leave much poorer evidence in these particular fossils than do teeth and jaws. Precise adult dental occlusion is easier to maintain when repeated replacement ceases. The lineage subsequently passed through Theria, Eutheria and the ancestors of living placental mammals. These nested relationships matter: a Cretaceous eutherian is not automatically a member of the living placental crown group, and neither the first known fossil nor the date of a tooth innovation fixes the origin of an entire group.
The immediate terrestrial context of whale evolution is within Artiodactyla, broadly circumscribed to include Cetacea. Living hippopotamuses are the closest living relatives of cetaceans, not their ancestors. Some early whale teeth suggested relationships with extinct mesonychians, but dental resemblance alone was misleading. Early whale skeletons preserve the characteristic artiodactyl double-pulley astragalus, providing a powerful independent anatomical test of the relationship inferred from molecular evidence. The relevant comparison is the detailed construction of the ankle, not simply whether an animal has hooves or eats meat. [ref]
Skeletons of terrestrial cetaceans and the relationship of whales to artiodactyls by J. G. M. Thewissen and others. Nature 413, pp. 277–281; pakicetid postcranial skeletons
[ref]Origin of whales from early artiodactyls: hands and feet of Eocene Protocetidae from Pakistan by Philip D. Gingerich and others. Science 293, pp. 2239–2242; protocetid ankle anatomy
Early Eocene pakicetids, roughly 50 Ma, combine a largely terrestrial, weight-bearing skeleton with diagnostic whale ear-region anatomy, notably the thickened medial wall of the auditory bulla called the involucrum. Thus identification as a whale does not imply an obligately marine animal. Ambulocetus, roughly 48 Ma, has a different combination: robust limbs still useful around shore, large feet and an axial skeleton suited to substantial movement in water. Reconstruction of amphibious locomotion uses limb proportions, joint surfaces and vertebral anatomy together; it does not require assuming that its swimming exactly resembled an otter's. These are successive grades represented by branching relatives, not proof that a particular pakicetid gave birth to the known Ambulocetus specimen. [ref]
From Land to Water: the Origin of Whales, Dolphins, and Porpoises by J. G. M. Thewissen and others. sections on pakicetids, ambulocetids, protocetids and basilosaurids
Middle Eocene protocetids further document reduction of terrestrial support and increasing commitment to swimming. Changes in the connection between pelvis and vertebral column, limb proportions and the position of external nostrils occurred in different combinations. The ankle of Rodhocetus is especially informative about ancestry even while other parts of its skeleton document aquatic specialization. It would be unjustified to draw a preserved tail fluke onto Rodhocetus: a reconstructed swimming mode must distinguish actual preserved anatomy from inferred soft parts. [ref]
Origin of whales from early artiodactyls: hands and feet of Eocene Protocetidae from Pakistan by Philip D. Gingerich and others. Science 293, pp. 2239–2242; protocetid ankle anatomy
Aquatic hearing changed alongside locomotion. Enlargement of the mandibular sound-reception region and changes in the middle ear support a transition towards receiving underwater sound through the lower jaw, with increasing acoustic separation of the ears from the skull. Early whale lineages display different intermediate combinations, so the presence of an involucrum alone does not imply a modern dolphin hearing system. Reconstructing soft sound-conducting tissues requires comparison with living anatomy; the fossil preserves their bony context rather than the entire pathway. [ref]
Eocene evolution of whale hearing by Sirpa Nummela and others. Nature 430, pp. 776–778; sound transmission reconstructed from early whale ear and jaw anatomy
By the later Eocene, basilosaurids were fully aquatic. The forelimbs functioned as flippers, the vertebral column and tail supplied propulsion, and the hind limbs were far too small to support terrestrial walking. Nevertheless, the reduced limbs of Basilosaurus retain recognizable limb and foot elements. Loss of a locomotor role is not equivalent to absence of all function; reproductive or muscular roles are compatible with reduction, although a specific behaviour cannot be read directly from a bone. The transition therefore involved changing proportions and connections as well as losses. [ref]
Hind limbs of Eocene Basilosaurus: evidence of feet in whales by Philip D. Gingerich and others. Science 249, pp. 154–157; reduced pelvis and hind limbs
Finally, the living branches acquired different specializations. Odontoceti retain teeth and evolved specialized sound production and echolocation; Mysticeti evolved baleen and lack functional adult teeth. fossil toothed mysticetes and degraded enamel-related genes show that modern toothlessness is derived. Palatal vascular features have been used to infer an intermediate combination of teeth and baleen, but such foramina do not preserve the baleen itself, and the exact sequence of feeding behaviours is less secure than the transition from toothed ancestry. [ref]
Morphological and molecular evidence for a stepwise evolutionary transition from teeth to baleen in mysticete whales by Thomas A. Deméré and others. Systematic Biology 57, pp. 15–37; palatal foramina, tooth characters and enamel-gene pseudogenes
The resulting history explains why a whale can have a mammalian jaw and reproductive system, an artiodactyl ancestry, a radically modified swimming skeleton, and a feeding apparatus that evolved after the aquatic transition. The strongest reconstruction combines nested anatomical characters with independently dated fossils, while treating soft-tissue and behavioural reconstructions as hypotheses.Repeated dietary adaptations reflect recurring mechanical and digestive demands, but a similar diet need not produce identical anatomy, and anatomical resemblance need not represent an independent evolutionary origin. A useful comparison places each example on a phylogenetic tree, identifies the inherited structure being modified, and separates food acquisition, oral processing and digestion.
Among dental adaptations, shearing blades recur in meat-eating mammals. In Carnivora, a placental order within Laurasiatheria, the main carnassial pair comprises the upper fourth premolar and lower first molar. Their opposing blades slice flesh, while relative development of crushing surfaces varies with diet. Predatory marsupials, including the extinct thylacine within Dasyuromorphia, also emphasize shearing, but do not reproduce precisely the same specialized tooth pair. The jaw and basic tooth classes are inherited mammalian structures; the highly blade-like feeding apparatus represents convergent evolution of performance in separate therian branches. Within Carnivora, resemblance between close relatives may instead reflect shared ancestry, and specialized insect-eating or plant-eating members demonstrate that membership of the order does not establish a carnivorous diet.
Repeated elaboration of grinding surfaces provides a complementary case. lophodonty joins tooth cusps into ridges, and selenodonty produces crescentic ridges, maintaining effective cutting edges as the surface wears. Herbivorous perissodactyls, including horses, contrast with ruminants such as bovids and cervids in Artiodactyla; both are within Laurasiatheria. Complex grinding teeth also evolved in proboscideans within Afrotheria and in macropods, a marsupial lineage within Diprotodontia. These positions rule out treating every complex herbivore tooth as one recent innovation inherited from a common grazing ancestor. Three-dimensional measurements of occlusal surface complexity in carnivorans and rodents show that dietary demands can produce comparable patterns across very different tooth constructions. The useful prediction concerns functional surface geometry, not identical cusp names in every group. [ref]
High-level similarity of dentitions in carnivorans and rodents by Alistair R. Evans and others. Nature 445, pp. 78–81; three-dimensional occlusal complexity and diet
Resistance to abrasion repeatedly modifies tooth growth as well as tooth shape. hypsodonty supplies a tall reserve crown that is progressively exposed by wear; it occurs in several ungulate groups and in some marsupials. It differs from hypselodonty, in which teeth continue growing, as in rodent incisors. Self-sharpening incisors, with uneven distribution of tooth enamel and differential wear of dental tissues, facilitate gnawing. Rodentia and Lagomorpha are both within Glires, so their incisor similarities must be analysed against that relationship rather than automatically counted as two independent origins of the whole dental system.
A high crown is a wear-management adaptation, not an infallible grass detector. Abrasive particles can come from vegetation or ingested external dust and grit; food toughness and abrasiveness are also distinct. North American horse fossils show substantial variation in dental mesowear within populations and temporal relationships between dietary abrasion and crown-height changes that are more complicated than an instantaneous switch from browsing to grazing. [ref]
Dietary Change and Evolution of Horses in North America by Matthew C. Mihlbachler and others. Science 331, pp. 1178–1181; mesowear compared with crown-height evolution
A defensible palaeodiet reconstruction combines tooth form with dental microwear, dental mesowear, stable isotope analysis where suitable, and environmental evidence. dental microwear emphasizes relatively recent meals, whereas crown form reflects inherited morphology across generations. Disagreement can therefore be informative rather than an analytical failure.A major non-dental recurrence is an enlarged gut compartment supporting microbial fermentation. mammals do not obtain the full energy value of structural plant carbohydrates through their own enzymes alone; microbial partners release usable fermentation products, notably short-chain fatty acids. foregut fermentation evolved in ruminants, colobine monkeys within Primates, and macropods. The forestomach compartments are not identical organs merely because each houses microbial digestion: the relevant independent changes concern enlargement, compartmentalization, retention and mixing in phylogenetically separated lineages. In ruminants, rumination additionally returns food for further mastication, increasing the surface available to microorganisms.
hindgut fermentation provides another solution. horses, within Perissodactyla, use enlarged caecal and colonic compartments; rabbits, within Lagomorpha, combine caecal processing with cecotrophy, reingesting selected soft material and thereby recovering microbial nutrients through a second passage. foregut fermentation allows microbial products and microbial biomass to encounter later digestive regions, whereas hindgut fermentation can accommodate high intake and rapid passage of some food fractions. Neither arrangement is universally superior: retention time, food quality, body size, intake rate and the ability to select particles affect the balance. The comparative explanation of equid success therefore requires throughput as well as percentage extraction from a single meal. [ref]
The evolutionary strategy of the Equidae and the origins of rumen and cecal digestion by Christine M. Janis. Evolution 30, pp. 757–774; retention, throughput and digestive strategies
Food acquisition supplies a further non-dental example. anteaters, within Xenarthra, and pangolins, within Pholidota in Laurasiatheria, independently combine reduction or loss of teeth with an elongated, protrusible tongue and a feeding apparatus suited to taking small social insects. Powerful forelimbs and claws can open nests, but digging also serves many other functions; claws alone do not identify ant feeding. Conversely, absence of grinding teeth need not signify nutritional simplicity: prey capture, protection from prey defences and microbial digestion can remain specialized.
Comparative dissection of primate digestive tracts supplies an independent anatomical test: gut compartments and their relative dimensions can be compared with diet rather than guessed from the teeth. Such comparisons must account for body size and the non-independence of related taxa. [ref]
Morphology of the gastrointestinal tract in primates: comparisons with other mammals in relation to diet by David J. Chivers and others. Journal of Morphology 166, pp. 337–386; comparative gut measurements and dietary categories
Testing these interpretations requires more than a gallery of look-alikes. Record diet in wild animals, compare anatomical performance under relevant loads, measure gut retention or digestive products, and include relatives with different diets. Control for body size, age, sex, tooth wear stage and shared ancestry, since ten related grazers are not ten independent evolutionary experiments. For fossils, preserve the distinction between direct anatomical observation and an inferred gut or behaviour. The repeated solutions are cutting or grinding surfaces, mechanisms that sustain those surfaces under wear, specialized acquisition structures and microbial digestive chambers; their phylogenetic distribution reveals both convergence and inherited constraints.Southern fossils have changed the geography, timing and anatomical character of mammaliaform evolution, while exposing how strongly a northern fossil record had shaped earlier expectations. Their importance is not that every southern lineage arose in the south. A dated occurrence establishes presence and a minimum age; an evolutionary origin requires an argument from phylogenetics and biogeography. Nor do modern continental outlines reproduce the connections of Gondwana.
A particularly consequential example is Ambondro mahabo, represented by a jaw fragment with lower teeth from Middle Jurassic Madagascar, approximately Ma. The teeth possess a basined heel associated with the crushing component of tribosphenic molars, which combine shearing and crushing in a single occlusal system. Its age extended the then-known record of this dental construction substantially backwards and challenged a simple northern origin inferred from better-sampled northern localities. The material nevertheless consists of a very restricted part of the animal, and the matching upper dentition was not directly observed. Assigning the entire skeleton, physiology or reproductive mode from these teeth would go beyond the evidence. [ref]
A Middle Jurassic mammal from Madagascar by John J. Flynn and others. Nature 401, pp. 57–60; Ambondro lower jaw, approximately 167 ± 2 million years old
The discovery also changed the character of the phylogenetic question. One hypothesis groups several southern forms in Australosphenida, associated with the ancestry of monotremes, and proposes that a tribosphenic-like construction arose independently of northern Boreosphenida, including therians. In that interpretation a highly functional tooth arrangement is convergent evolution, not a unique certificate of therian ancestry. A competing analysis supports a single origin of tribospheny and rearranges the relationships of the relevant southern taxa. [ref]
Dual origin of tribosphenic mammals by Zhe-Xi Luo and others. Nature 409, pp. 53–57; alternative placements of southern tribosphenic mammals
[ref]The evolution of tribospheny and the antiquity of mammalian clades by Michael O. Woodburne and others. phylogenetic analysis supporting a single origin of tribospheny
The important lesson is not to declare one historical topology established by the striking tooth alone. The choice depends on which cusps and basins are judged instances of biological homology, character coding, inclusion of other anatomical regions, and the taxon sample. Nor does a Middle Jurassic tribosphenic tooth by itself date the split between living marsupials and placental mammals.South American monotreme material further undermined the equation of present distribution with evolutionary birthplace. Early Paleocene Monotrematum, approximately 60–65 Ma, has teeth with affinities to the platypus lineage. Living monotremes are restricted to Australasia, but that restriction cannot be projected unchanged into the past. [ref]
First discovery of monotremes in South America by Rosendo Pascual and others. Nature 356, pp. 704–706; Paleocene Monotrematum teeth
South America, Antarctica and Australia offered changing opportunities for connection, fragmentation and movement. A South American occurrence is compatible with a geographically extensive southern history; it does not uniquely establish the direction of dispersal or prove that Monotrematum was the direct ancestor of the living platypus. The distinction between a crown group and related members of its stem group is essential when attaching such fossils to divergence-time estimates.Latest Cretaceous Madagascar has contributed more than isolated tooth surprises. The cranium of Vintana, around 70 Ma, supplied extensive new characters for the formerly tooth-dominated Gondwanatheria. Its robust feeding apparatus and unusual cranial combination permit tests of relationships and ecology that were unavailable from a few teeth. Yet a mosaic of familiar and unusual features is precisely the situation in which a single apparently diagnostic character can mislead. The placement of gondwanatherians therefore needs broad anatomical and taxonomic comparison, including other extinct groups, rather than assignment to a living order by superficial resemblance. [ref]
First cranial remains of a gondwanatherian mammal reveal remarkable mosaicism by David W. Krause and others. Nature 515, pp. 512–517; Vintana cranium and phylogenetic character sampling
The approximately 66 Ma skeleton of Adalatherium expanded that evidence into the postcranial skeleton. It documents a relatively large, several-kilogram non-therian mammal with an unusual combination of cranial, dental, vertebral and limb features. This contradicts the caricature that all Mesozoic mammaliaforms were anatomically interchangeable tiny insect-eaters. Madagascar's long isolation provides a plausible context for its evolutionary distinctiveness, but the claim that isolation caused a particular feature remains an explanatory hypothesis. One needs comparative island and continental samples to distinguish an island effect from inherited lineage-specific anatomy. [ref]
Skeleton of a Cretaceous mammal from Madagascar reflects long-term insularity by David W. Krause and others. Nature 581, pp. 421–427; Adalatherium skeleton and insularity hypothesis
Australia's early Eocene Djarthia, approximately 55 Ma, addresses a different issue: the relationships and movement of marsupials. Its ankle material supports a position close to the base of Australidelphia, a group containing the living Australian orders and the South American Microbiotheria. This is stronger evidence than assuming that every small Australian jaw belongs inside a modern Australian family. [ref]
Australia's Oldest Marsupial Fossils and their Biogeographical Implications by Robin M. D. Beck and others. PLoS ONE 3, e1858; Djarthia tarsals and australidelphian relationships
It is compatible with a history involving South America and Antarctica, but a branching order is not a map of a single migration. An extinct distribution can be extensive, intermediate populations can disappear, and the oldest sampled fossil need not occur near the place where a lineage originated. Also, the older and more inclusive Metatheria must not be confused with the living marsupial crown group.Together these discoveries change how large-scale history is tested. First, expanding southern sampling can overturn a supposed absence that arose from collecting intensity, exposure of suitable rocks or preservation. taphonomy and the concentration of many early records on durable teeth must be modelled before comparing continental diversity. Second, new skeletons can change the inferred phylogenetic tree, and therefore whether a tooth adaptation counts as one origin or several. Third, fossil calibration constrains the minimum age of a lineage, with explicit uncertainty in both geological age and phylogenetic assignment. Fourth, continental drift changes which dispersal routes were physically plausible. Shared distributions across former Gondwana may reflect vicariance, later dispersal, or a mixture; the geological separation must be compared with a defensible lineage age rather than used as its automatic explanation.
From the Jurassic through the Palaeogene, these independent discoveries have cumulatively changed both the anatomical evidence and its interpretation. They reveal a more diverse southern mammaliaform history and force explicit tests of convergence, missing data and geographic sampling, rather than replacing an assumed northern centre with an equally assumed southern centre.
Repeated movements out of Africa are compatible with a predominant shared source for the ancestry of living non-Africans. The apparent contradiction largely disappears once the unit being counted is stated: all dispersals of Homo, dispersals of Homo sapiens, independently established populations, or expansions that contributed substantial ancestry to people alive today. These are different historical claims.
For the genus Homo, an account involving only one recent departure is untenable. Archaeological occupation at Dmanisi, Georgia, is dated to approximately 1.85–1.78 Ma, long before the late Pleistocene expansion of Homo sapiens. The earliest occupation levels must be distinguished from the somewhat younger hominin-bearing deposits: the site is not a single instantaneous event. Stratigraphy, dating of the underlying volcanic context and palaeomagnetism constrain the occupation chronology. [ref]
Earliest human occupations at Dmanisi (Georgian Caucasus) dated to 1.85–1.78 Ma by Reid Ferring and others. Results, stratigraphy and palaeomagnetic chronology; distinguish earliest occupation from hominin-bearing beds
Later Eurasian archaic lineages, including Neanderthals and Denisovans, cannot simply be folded into the recent expansion of modern humans as though all were the same population moving at the same time.Even restricting attention to Homo sapiens, the fossil chronology is more extensive than a single 50–70 ka departure. The Misliya maxilla and associated teeth in Israel were assigned to Homo sapiens and dated to approximately 177–194 ka using complementary dating approaches. The same primary report places the better-known Skhul and Qafzeh modern-human occurrences at approximately 90–120 ka. [ref]
The earliest modern humans outside Africa by Israel Hershkovitz and others. Science 359, pp. 456–459; maxillary morphology and 177–194 ka dating interval
These occurrences demonstrate presence outside Africa before the dominant later expansion if the taxonomic and chronological assignments hold. They do not by themselves demonstrate uninterrupted occupation, a particular migration route through Arabia, or a large surviving genetic contribution to present-day Eurasians.Apidima adds an important but less secure claim. Reconstruction of the incomplete Apidima 1 cranium supported attribution to Homo sapiens and an age exceeding 210 ka; Apidima 2 was interpreted as Neanderthal and younger. [ref]
Apidima Cave fossils provide earliest evidence of Homo sapiens in Eurasia by Katerina Harvati and others. Nature 571, pp. 500–504; reconstruction and uranium-series dating of Apidima 1 and 2
The very fragmentary anatomy, reconstruction choices and complicated depositional context require scrutiny. An assigned minimum age is not an exact date of arrival, and a different reconstruction or taxonomic diagnosis can alter the biogeographic inference. The sensible argument for early departures therefore uses the converging set of dated remains and its uncertainty, rather than treating the oldest proposed specimen as a decisive, uncontested fact.The main evidence favouring a single principal source is genetic. Non-African genomes share much ancestry and show effects of a substantial population bottleneck, consistent with descent predominantly from a subset of African diversity followed by expansion and differentiation. Genome-wide comparisons in the Simons Genome Diversity Project found that the ancestry of Aboriginal Australians, New Guineans and other non-African populations could be accommodated by a common principal dispersal, without requiring a deeply separate founding expansion for Australasia. [ref]
The Simons Genome Diversity Project: 300 genomes from 142 diverse populations by Swapan Mallick and others. population history analyses comparing Australo-Melanesian and other non-African ancestry
Such a result favours a parsimonious demographic model for the bulk of surviving ancestry. It does not observe a unique group crossing a border on one date, nor rule out movements whose descendants disappeared.Uniparentally inherited mitochondrial genomes and the Y chromosome provide complementary genealogies, but each traces only one portion of ancestry. Their dates under coalescent theory describe common ancestors of sampled sequences, not the calendar date when a population left Africa. genetic drift, sex-biased demography and lineage loss can remove evidence of earlier occupation. Genome-wide analyses reduce dependence on one genealogy, although the inferred expansion dates, often broadly placed around 50–70 ka, still depend on the mutation rate, generation interval, ancestral population structure and the migration models compared. A prolonged connected expansion can resemble one founder event in a simplified model.
There is also genetic evidence that complicates an absolute single-expansion claim. One analysis inferred a small contribution to Papuan ancestry from an earlier expansion, while still attributing the great majority of non-African ancestry to a shared later expansion. [ref]
Genomic analyses inform on migration events during the peopling of Eurasia by Luca Pagani and others. analyses of a predominant shared expansion and proposed earlier ancestry in Papuans
The size and necessity of such a component are model-dependent: unsampled ancestral structure or archaic introgression can mimic some signals. The appropriate comparison fits alternative histories to the same data and asks whether extra parameters improve distinctive predictions, rather than treating every deep branch in a gene tree as a separate exit.Archaic admixture makes the ancestry history explicitly reticulate. Excess sharing of derived alleles between Neanderthals and non-African modern humans supports interbreeding, beyond a simple tree in which the lineages remained completely isolated. [ref]
A draft sequence of the Neandertal genome by Richard E. Green and others. Science 328, pp. 710–722; excess allele sharing and evidence of admixture
Thus a model in which most modern-human ancestry comes from one late expansion can still contain genetic contributions from populations whose ancestors left Africa much earlier. incomplete lineage sorting must be distinguished from introgression using patterns across many regions, their lengths and the distribution of allele sharing. Back-migration into Africa further prevents “African” and “non-African” from being permanently sealed categories.Africa itself should not be represented as a homogeneous ancestral village. Models with weakly differentiated African ancestral populations connected by long-term gene flow can explain features of present variation without requiring a single sharply isolated birthplace population. [ref]
A weakly structured stem for human origins in Africa by Aaron P. Ragsdale and others. Nature 617, pp. 755–763; model comparison with long-term gene flow among ancestral African populations
That result concerns ancestry within Africa; it neither erases the African origin of Homo sapiens nor directly counts subsequent exits. Geographically, northern routes through the Levant and southern routes through Arabia remain testable alternatives or complements. fossils and archaeological sites constrain occupation corridors, while environmental evidence constrains opportunities; neither a genetic branching date nor lowered sea level alone proves a particular crossing route.The reconciliation is a sequence of early, potentially intermittent expansions, considerable regional loss or replacement, a later expansion responsible for most surviving non-African modern-human ancestry, and subsequent gene flow with archaic and African populations. Testing it requires directly dated remains, secure taxonomic comparisons, independent genetic samples, explicit demographic alternatives and allowance for unsampled populations. “One dominant ancestry expansion” is a much narrower and better-supported proposition than “only one movement out of Africa”; multiple movements need not imply several equally large surviving founding ancestries.
Living great apes are indispensable comparative evidence, but none is a preserved version of the Pan–Homo last common ancestor. The ancestor was a population with its own combination of traits, and every living descendant has subsequently evolved. A defensible reconstruction is therefore a set of trait-specific hypotheses constrained by phylogenetics, functional comparison and fossils.
The comparison starts with relationships. Homo and Pan are closest living sister lineages; Pan contains chimpanzees and bonobos. Gorilla provides a more distant comparison, and Pongo a more distant one again. Humans are themselves great apes, rather than a group standing outside them. A character shared by Pan and Homo may have been inherited from their last common ancestor, but it can also have changed in either lineage or arisen in parallel. A shared feature of Pan and Gorilla does not automatically reconstruct the ancestor either: it may be ancestral, convergent, or retained in some branches and lost in others.
Living great apes are especially valuable because their soft tissues, growth, behaviour and mechanical performance can be studied. Muscle paths, joint motion and hand loading can make competing functional interpretations of a fossil wrist testable. Observing climbing and terrestrial movement establishes which combinations are mechanically possible; it also exposes the inadequacy of labelling a whole animal simply “arboreal” or “terrestrial”. Appropriate controls compare individuals of different ages and sexes, adjust for body size, record substrate and loading, and distinguish performance in captivity from behaviour in the wild. A surface that resembles another surface is weak functional evidence unless its position in the complete joint and the range of loads are considered.
The same accessibility creates temptations. chimpanzee locomotion, male coalitions or territorial behaviour cannot be transferred wholesale to the common ancestor. bonobos demonstrate variation within Pan, not a second unchanged ancestral template. Ecology, group composition, developmental plasticity and histories of selection differ among living populations. Current behaviour can generate hypotheses about feasible ancestral social systems, but proving that a particular ancestral behaviour existed requires additional evidence; most social behaviours do not fossilize. Treating the contrast as a choice between a uniformly aggressive chimpanzee ancestor and a uniformly peaceful bonobo ancestor replaces biology with caricature.
knuckle-walking illustrates the genuine scientific alternatives. One reconstruction takes the shared use of knuckle support in Pan and Gorilla as evidence for an ancestral condition, with later loss or modification in the hominin lineage. wrist features in early hominins have been interpreted as retained support for that hypothesis. [ref]
Evidence that humans evolved from a knuckle-walking ancestor by Brian G. Richmond and others. Nature 404, pp. 382–385; wrist characters interpreted as retained knuckle-walking adaptations
A competing study emphasized differences in the development and functional organization of chimpanzee and Gorilla wrists, consistent with independent origins of their knuckle-walking systems. [ref]Independent evolution of knuckle-walking in African apes shows that humans did not evolve from a knuckle-walking ancestor by Tracy L. Kivell and others. PNAS 106, pp. 14241–14246; contrasts between chimpanzee and gorilla wrist development and function
Similar external posture can therefore conceal distinct load-bearing arrangements. Neither simply counting two living knuckle-walking genera nor quoting the conclusion of one comparative study settles the ancestral condition. The inference depends on biological homology, functional interpretation and inclusion of relevant extinct forms.Ardipithecus ramidus, approximately 4.4 Ma, is particularly important because its skeleton combines a grasping great toe and arboreal capabilities with anatomy interpreted as supporting terrestrial bipedalism. The authors argued that its hands and feet did not represent an unchanged modern chimpanzee locomotor package. [ref]
Ardipithecus ramidus and the paleobiology of early hominids by Tim D. White and others. Science 326, pp. 75–86; 4.4 Ma skeleton and locomotor mosaic
This weakens a reconstruction that derives early hominins by merely standing a modern chimpanzee upright. However, Ardipithecus lived after the inferred Pan–Homo divergence; its features may include specializations of its own. Its proposed hominin position and functional reconstruction must also be evaluated against incomplete preservation and distortion, especially in the pelvis. It is evidence about a nearby branch, not direct observation of the common ancestor.Older Miocene apes extend the comparison beyond surviving lineages. Pierolapithecus, approximately 12.5–13 Ma, combines an upright-trunk construction (orthogrady) with hand anatomy lacking the complete suspensory specialization of some living apes. [ref]
Pierolapithecus catalaunicus, a new Middle Miocene great ape from Spain by Salvador Moyà-Solà and others. Science 306, pp. 1339–1344; orthograde trunk and contrasting hand morphology
The example shows that trunk posture, climbing and suspensory locomotion can evolve as a mosaic. Its exact position is debated, and it is not thereby identified as the Pan–Homo ancestor. Rather, extinct combinations expand the set of plausible ancestral forms and can reveal that a feature widespread among living apes was assembled in stages.Genetic evidence establishes relationships and helps constrain timing, but a molecular divergence estimate is not a fossil anatomical reconstruction. Estimates are sensitive to mutation rate, calibration and generation interval. Pedigree observations of wild chimpanzees and Gorilla demonstrate why substituting one universal generation length can shift the inferred dates of great-ape divergences. [ref]
Generation times in wild chimpanzees and gorillas suggest earlier divergence times in great ape and human evolution by Kevin E. Langergraber and others. PNAS 109, pp. 15716–15721; pedigrees, generation intervals and divergence-time sensitivity
A gene tree can also coalesce before a population split, and incomplete lineage sorting means that not every genomic region follows the species branching order. There is consequently no reason to force every candidate fossil into an overly precise split date selected from one molecular estimate.The best procedure is to specify competing ancestral states and their predictions: for example, whether a particular wrist character should accompany habitual knuckle support, or whether an inferred climbing apparatus requires suspensory finger proportions. Score those characters across Pan, Homo, Gorilla, Pongo and well-preserved fossil taxa; examine sensitivity to uncertain character coding and alternative fossil placements. Related features must not be counted as a large number of independent confirmations when they are mechanically or developmentally coupled. Extant-only ancestral state reconstruction is especially vulnerable to the extinction of lineages that possessed combinations absent today.
Living great apes supply the comparative mechanics, development and diversity needed to interpret fossils; fossils prevent the living sample from dictating a false ancestral stereotype. A cautious composite reconstruction, with separate uncertainty for posture, hand use, diet and behaviour, is more defensible than choosing one living species as the ancestor's complete anatomical and social model.
The Holocene history combines natural climatic and geographic filtering with increasingly strong human restructuring through hunting, habitat change, domestication, introductions and conservation. The balance varies through time and between Britain and Ireland. The Holocene begins approximately 11.7 thousand calibrated years before present; for radiocarbon dating, “present” conventionally means 1950. Uncalibrated radiocarbon ages must not be silently treated as calendar ages.
At the beginning, warming following the last glaciation changed vegetation and the distribution of food and cover. Open, cold-adapted assemblages gave way to a changing mixture of woodland, wetland and open-habitat mammals. Rising seas progressively restricted natural colonization; Britain retained connections to continental Europe later than Ireland's faunal assembly can simply be assumed to have done. The modern Irish fauna is therefore not a complete British fauna subsequently pruned by identical extinctions. A missing Irish species may never have colonized, rather than having been exterminated there. pollen analysis, stratigraphy and directly dated bones help distinguish habitat change from collecting gaps.
Chronology prevents an equally misleading division into wholly “Pleistocene” losses and wholly modern survivors. Some conspicuous cold-stage mammals, such as the woolly rhinoceros, disappeared from Britain before the Holocene and should not automatically be included in a Holocene hunting-extinction list. Conversely, directly dated giant deer from the northern Irish Sea basin demonstrate early Holocene survival of a lineage once thought to have disappeared regionally earlier. [ref]
Survival of the Irish elk into the Holocene by Silvia Gonzalez and others. Nature 405, pp. 753–754; directly dated giant deer from the northern Irish Sea basin
A date from one part of this region does not establish persistence everywhere in Ireland or Britain. Local disappearance, regional disappearance and global extinction are different endpoints; environmental deterioration and human activity need to be evaluated at the appropriate geographic and chronological scale.Later prehistory saw a profound change in mammalian abundance as farming spread. Domestic cattle, sheep, goats and pigs became major components of archaeological assemblages and living biomass. Grazing, clearance and woodland management altered habitat for wild herbivores and their predators; settlement and stored food also favoured commensal rodents. This was more than adding several species to an unchanged ecosystem. Distinguishing domestic from wild forms requires skeletal comparisons, context and, where available, Ancient DNA and stable isotope analysis. A large number of livestock bones in a settlement midden is evidence of human use, not a direct census of every mammal in the surrounding landscape.
Losses of large native species were staggered. British aurochs, wild boar, lynx, brown bears, beavers and wolves disappeared at different times through combinations of hunting, persecution, habitat transformation and habitat fragmentation. The list cannot be transferred intact to Ireland: a secure native record must be established for each taxon, and a late imported specimen does not demonstrate an earlier indigenous population. Small and elusive species are also less visible in many archaeological deposits, so the absence of their remains should not be equated with a known extinction date.
The dated British lynx record is especially instructive. Survival into the early medieval period makes an explanation based solely on warming at the start of the Holocene inadequate. Human habitat change and direct or indirect persecution become more plausible proximate causes, although the last dated specimen cannot identify which pressure killed the final population. [ref]
New evidence for the occurrence of Eurasian lynx (Lynx lynx) in medieval Britain by David A. Hetherington and others. Journal of Quaternary Science 21, pp. 3–8; directly dated lynx bone and implications for extinction causes
brown bear history is less tidy: review of the British evidence supports either late Neolithic/early Bronze Age or early medieval extinction, and later archaeological bear remains can represent imported captive animals rather than surviving wild populations. [ref]The presence of the brown bear Ursus arctos in Holocene Britain: a review of the evidence by Hannah J. O'Regan. assessment of native survival versus imported animals and alternative extinction chronologies
Traditional stories of the “last wolf” likewise require caution; historically documented persecution is much stronger evidence of human pressure than an unverified exact last-kill year.Human transport makes apparent continuity equally uncertain. Combined skeletal, Ancient DNA and phylogeography evidence indicates a complex Irish red deer history involving prehistoric and recent introductions, rather than simple uninterrupted survival of every modern population from the last glaciation. Neolithic-era records and the contrast between older Kerry-associated ancestry and many recent stocks must be interpreted with sampling gaps in mind. [ref]
Phylogeographic, ancient DNA, fossil and morphometric analyses reveal ancient and modern introductions of a large mammal: the complex case of red deer (Cervus elaphus) in Ireland by Ruth F. Carden and others. Quaternary Science Reviews 42, pp. 74–84; Neolithic record, ancient DNA and recent introductions
Modern distribution alone cannot distinguish an ancient native population, an early species translocation, and a recent estate introduction. Each may require a different conservation interpretation even if all animals bear the same species name.fallow deer provide a clearer example of deliberate species translocation. Integrated archaeological and biomolecular research traces Roman movements and later medieval redistribution, including the British history of introduction and reintroduction. [ref]
The 10,000-year biocultural history of fallow deer and its implications for conservation policy by Karis H. Baker and others. British Roman introductions and medieval translocations; combined biomolecular and archaeological evidence
Managed rabbits and later introductions of sika deer, muntjac, grey squirrels and American mink further altered assemblages. Some escaped from breeding or management; others were deliberately released. Historical records establish routes and timing that cannot be deduced from climatic suitability alone. Modern invasions are thus a continuation of human-mediated assembly, with potentially stronger effects because transport crosses barriers that once limited colonization.The replacement of red squirrels by grey squirrels illustrates multiple interacting mechanisms. interspecific competition for resources can matter, but experimental infection demonstrated severe infectious disease in red squirrels with little detectable effect on grey squirrels, supporting a role for squirrelpox in some declines. [ref]
Parapoxvirus causes a deleterious disease in red squirrels associated with UK population declines by Daniel M. Tompkins and others. Proceedings of the Royal Society B 269, pp. 529–533; contrasting experimental susceptibility of red and grey squirrels
That experiment establishes differential susceptibility; it does not show that every field decline is caused by the virus. A field test must establish infection exposure as well as squirrel abundance and account for habitat and competitor density. Likewise, recovery of pine martens in Ireland has been associated with declines of grey squirrels and recovery opportunities for red squirrels; the evidence is informative but a spatial association alone is not a controlled demonstration that predation explains every local change. [ref]Population crash in an invasive species following the recovery of a native predator: the case of the American grey squirrel and the European pine marten in Ireland by Emma Sheehy and others. Biodiversity and Conservation 23, pp. 753–774; distributional changes associated with pine marten recovery
Recent protection, woodland recovery and reintroductions also allow people to reverse some earlier losses. Such recoveries do not recreate a unique pristine baseline: a “native” reference chosen at the beginning of the Holocene, before farming, or before modern introductions gives different assemblages. The same applies to interpreting recovering coastal populations; marine and terrestrial records need their own detection and exploitation histories. Reliable attribution combines directly dated remains, habitat evidence, historical documentation and demographic or experimental tests, with explicit allowance for preservation and survey effort.
Climate and access strongly shaped early Holocene assembly; later changes increasingly reflect farming, persecution and transport, with modern infectious disease and conservation adding further layers. Human influence is therefore pervasive, but neither every absence nor every change in abundance can be assigned to humanity without establishing when and where the change occurred.
The strength of conflicting interests, opportunities for exploitation and receiver defences matter more than the species boundary itself. Many striking examples occur between species, where shared descent usually supplies little inclusive fitness restraint. However, competition for mates and resources also creates substantial conflict within a species, including between relatives. The available examples do not establish a universal numerical ranking of the two settings.
A useful distinction is between deceptive signalling and the broader category of behavioural manipulation. A deceptive display exploits a receiver response in a context in which that response no longer provides the normally associated benefit. Manipulation also includes changing another organism's physiology or behaviour without conveying misleading information. Neither definition requires conscious lying or knowledge of another individual's beliefs. Ordinary persuasion is not a helpful biological criterion: the relevant comparison is between the reproductive success consequences for sender and receiver, relative to appropriate alternatives.
Between species, exploitation can borrow a response that is maintained for another reason. A predator can mimic an attractive prey cue; a parasite can exploit a host's provisioning or avoidance mechanism; and a plant can attract a pollinator without providing the expected reward. Such interactions can favour sensory exploitation and aggressive mimicry. Receiver resistance is selected when the losses outweigh its costs, but resistance need not eliminate deception. Rejecting a genuine mate or ignoring a real predator can be more costly than occasionally accepting a false signal.
In fork-tailed drongos, observations and playback experiments showed that false alarm calls can make other foragers abandon food, which the drongo steals. Receivers habituated to repeated alarms, while switching among alarm types, including mimicked calls, helped sustain responses. This demonstrates both an exploiter benefit and a receiver counterresponse. It does not require an inference that drongos attribute beliefs to their victims.[ref]
Deception by Flexible Alarm Mimicry in an African Bird by Tom P. Flower and others. 2014, field observations and playback tests of alarm variation and habituation
A different mechanism occurs in the orchid Ophrys sphegodes. Chemical analyses and behavioural tests implicated a floral blend matching components of female Andrena nigroaenea sex pheromone in attracting males that transfer pollen during attempted mating. Here deception exploits a reproductive response maintained in the pollinator's own species, rather than a communication system jointly serving orchid and bee. The orchid example demonstrates a specific mechanism, not the frequency of deception across all pollination systems.[ref]
Orchid pollination by sexual swindle by Florian P. Schiestl and others. 1999, floral chemistry and field behavioural tests
Behavioural manipulation can go beyond signals. In experimental comparisons, Toxoplasma gondii-infected rats showed altered responses to cat-associated odours, sometimes approaching locations avoided by uninfected rats. This is consistent with a transmission-enhancing effect because felids are the parasite's definitive hosts. However, an odour preference assay does not itself demonstrate increased predation by cats, greater parasite transmission, or that every infection-associated behavioural change is an adaptation. Illness, host defence and collateral pathology remain alternative explanations requiring separate tests.[ref]
Fatal attraction in rats infected with Toxoplasma gondii by M. Berdoy and others. 2000, experimental odour responses and interpretation
Within species, common ancestry does not imply identical interests. A mating partner may benefit from extra copulations that impose costs on the other partner; competitors may benefit by concealing food or exaggerating fighting ability; offspring may demand more care than maximizes parental lifetime reproductive success. Kin selection weakens some conflicts because harming a relative can also reduce an actor's inclusive fitness, but it does not generally remove them. For an unrelated rival, even that indirect cost may be absent.
Male topi provide a direct counterexample to the claim that deceptive communication is mainly possible across species. Field observations and playback work associated false alarm snorts with retaining receptive females within male territories and obtaining mating opportunities. Alarm responsiveness remains useful to females when a predator really is present, allowing a sexual conflict to exploit an otherwise protective response. The relevant opposition is male versus female mating interests, despite their membership of the same species.[ref]
Male Topi Antelopes Alarm Snort Deceptively to Retain Females for Mating by Jakob Bro-Jørgensen and Wiline M. Pangle. 2010, alarm context, female responses and mating consequences
There are also reasons why repeated interactions can restrain exploitation in either setting. A receiver can learn, recognize individuals, stop responding, abandon a partner, or impose a cost on it. In many mutualisms, both parties gain from preserving the association, even though each would benefit from obtaining more while supplying less. Conversely, within-species relatedness need not be high, and a short-lived encounter may give little opportunity for retaliation. Thus “between species” is an imperfect proxy for the underlying distribution of benefits, costs, encounter rates and alternatives.
To establish comparative prevalence, one would need a denominator: deceptive acts per interaction, the fraction of signal types exploited, the proportion of individuals using manipulation, or the number of independent evolutionary origins. Those measures can rank systems differently. Sampling would also need to control for observation effort, interaction frequency, detection probability and phylogenetic nonindependence. A concealed false signal can be harder to identify than an obvious parasite-induced change; spectacular cases attract disproportionate study.
The defensible prediction is conditional. Exploitation should be favoured where it increases the actor's reproductive success, the receiver's defences are ineffective or costly, and countervailing relatedness or future-interaction costs are small. Interspecific antagonism often meets these conditions, but so do some intraspecific sexual and competitive interactions. A comparative answer should therefore explain those conditions and acknowledge that the examples alone cannot settle a universal prevalence claim.
Both conflicts arise because family members value the same resource differently, but they concern different decisions. Sibling rivalry concerns allocation among offspring, whereas parent-offspring conflict concerns a parent's allocation relative to what an offspring would favour. Their consequences interact: offspring compete with one another inside a parental provisioning system that their own demands can also alter.
The basic mechanism is unequal genetic relatedness to the beneficiaries of an action. An offspring values its own additional survival or reproduction more strongly than an equal gain to a sibling. A parent, under a simple symmetric pedigree, is equally related to each of its offspring and can favour an allocation that maximizes their combined contribution. Neither statement implies that an offspring should demand everything: diverting resources from relatives can reduce its inclusive fitness. These differing interests underlie the original theory of parent-offspring conflict.[ref]
Parent-Offspring Conflict by Robert L. Trivers. 1974, theory of investment, sibling costs and the duration of care
Consider an explicit illustrative model. Let investment produce a direct offspring benefit and an opportunity cost measured in lost equivalent fitness contributions of other offspring. Assume a single parent, equal value of current and future offspring, no inbreeding, and relatedness between the focal offspring and those losing resources. After dropping a common parental relatedness factor, the parent's objective is , whereas the offspring's is . Interior optima therefore satisfyWith diminishing marginal benefits and , the offspring typically favours more investment. In particular, the range contains increments favoured by the offspring but opposed by the parent. For full siblings under the stated pedigree, ; for maternal half-siblings, . These values are not universal constants for all family structures, and parent survival, reproductive value and density dependence can alter the effective costs.
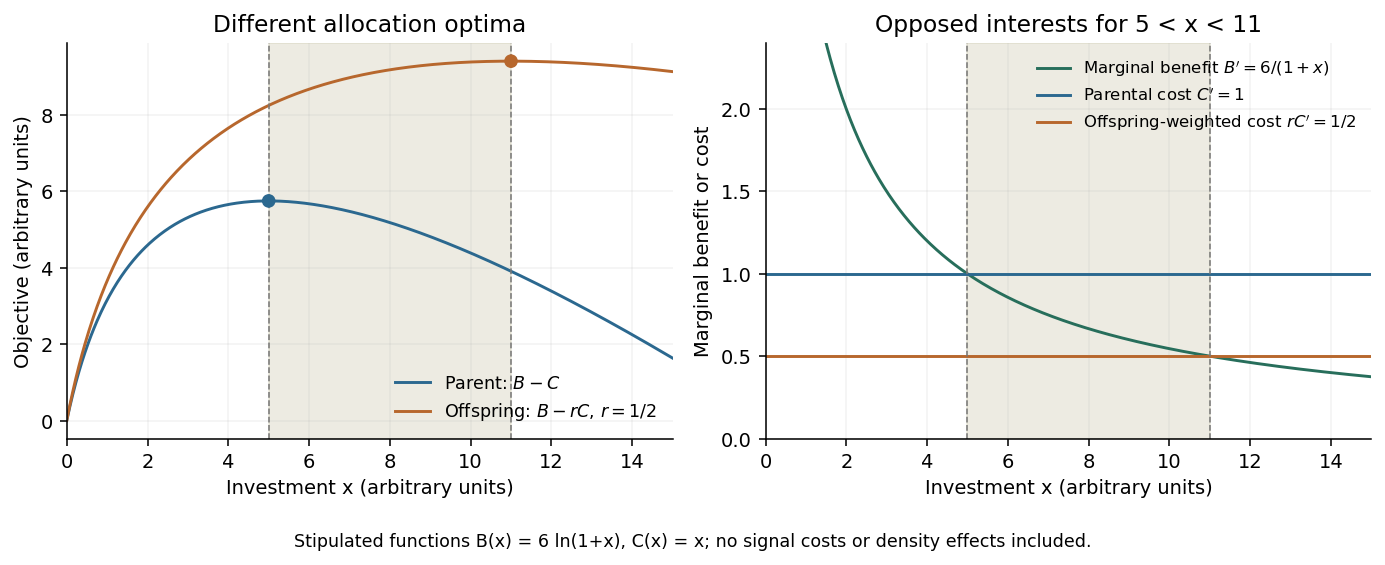
An original illustrative allocation model separates parental and offspring optima
. Chosen functions and give a parental optimum at and a full-sibling-weighted offspring optimum at . The shaded interval contains increments whose marginal benefit is below the parental opportunity cost but above the offspring-weighted cost. These are stipulated functions and arbitrary units, not empirical measurements. Details.
Sibling rivalry selects on relative access; parent-offspring conflict can also change the total supply. If one nestling obtains a larger fraction of a fixed food delivery, its sibling loses directly. Selection can favour size advantages, advantageous positions, earlier hatching or more effective solicitation. Severe asymmetries can permit siblicide or brood reduction. By contrast, a stronger demand directed at a parent can increase food delivery to the brood, potentially benefiting siblings too. The same begging behaviour can therefore redistribute a fixed supply and alter parental effort, with different consequences in each case.
A parent's preferred distribution need not be equal. A marginal food item may produce more surviving descendants when given to a smaller hungry chick, or to a larger chick that alone can survive a severe shortage. Parental allocation can consequently mitigate sibling asymmetry in one environment and reinforce it in another. Asynchronous hatching and brood-size adjustment are plausible parental means of structuring that contest; whether a particular asymmetry is an adaptation, a constraint or an offspring-driven outcome needs evidence. A parent's tolerance of brood reduction is not proof that every aggressive act serves parental interests.
Over evolutionary time, sibling rivalry can affect competitive morphology, growth schedules, solicitation, nest position and the survival distribution within broods. Parent-offspring conflict can affect the amount and duration of care, offspring demand, parental responsiveness, weaning schedules and the trade-off between current and future reproduction. Neither conflict predicts unlimited escalation. Energetic expenditure, injury, predation risk and losses to relatives can make competitive effort costly even when it obtains a larger resource share.
Information can produce compromise as well as waste. An offspring usually has private information about its hunger, while the parent integrates brood condition with its own prospects. In a costly-signalling model, offspring in greater need gain more from additional resources, so differing incentives can support informative solicitation at equilibrium. Such a result is conditional on the cost and benefit functions; it does not mean all begging is perfectly honest or that energetic expenditure alone establishes honesty.[ref]
Signalling of need by offspring to their parents by H. C. J. Godfray. 1991, primary signalling model and its assumptions
Signals can also be aimed at siblings. Experiments on barn owls found that nestlings reduced vocalization when a rival was hungrier, increased it after that rival was fed, and altered calling with experimental brood size. These calls occurred when parents were absent. They support sibling negotiation: assessing relative willingness to contest a future prey item can avert some unnecessary escalation. The experiment therefore cautions against treating every nestling call as a demand directed at the parent.[ref]
Barn owl (Tyto alba) siblings vocally negotiate resources by Alexandre Roulin and others. 2000, hunger and brood-size manipulations
A further consequence is coevolution among parental and offspring response rules. A demand phenotype expressed in young becomes part of the selective environment of provisioning adults, while parental allocation changes the returns to offspring competition. The same individual can experience both roles at different life stages, and genetic correlations between demand and care can constrain independent optimization. Thus observed care can be a compromise maintained by interacting strategies rather than the optimum of either party in isolation.
The comparison is consequently about overlapping arenas of selection. Sibling rivalry chiefly determines who obtains care, while parent-offspring conflict also determines how much care is supplied and when it ends. Both can generate competitive adaptations and costs, but both can also generate assessment, contingent responses and restraint. A strong empirical test must separate changes in total provisioning from redistribution, measure lifetime consequences rather than only immediate feeding success, and manipulate relatedness or information without simultaneously changing need.
Consistent individual differences can bias who leads, works, reproduces or takes risks, but a social role is usually produced jointly by an individual's traits and its social environment. A stable pattern of participation is not necessarily a fixed genetic caste, and observed specialization is not automatically evidence of superior skill.
First distinguish the measurements. Animal personality denotes repeatable among-individual differences in behaviour; a behavioural syndrome is a correlation across behavioural contexts. A social role describes an individual's contribution or position in a particular group, such as initiating travel or carrying brood. A member can repeatedly occupy a role because of morphology, age, nutritional state, information, experience or treatment by others. Some of these causes change predictably during life, so consistency over a short observation window need not imply lifelong specialization.
One proximate route is variation in behavioural response thresholds. A worker with a lower threshold for responding to brood demand begins care sooner; a hungry fish leaves shelter sooner; an informed animal initiates movement toward food. Once a member acts, it can reduce the stimulus facing others. That negative feedback helps partition labour even when initial differences are small. Conversely, practice or social reinforcement can lower the actor's future threshold or increase others' reliance on it, amplifying small initial differences into persistent roles. These are testable mechanisms, not reasons to assume that a group allocates tasks deliberately.
Animal leadership illustrates the importance of relational effects. In experimental pairs of three-spined sticklebacks, researchers first measured willingness to leave cover, then paired fish and modelled their movements. Relatively bold fish more often initiated joint trips, but both partners adjusted to the other's movements. Leadership therefore arose from differences in responsiveness as well as spontaneous initiation. It was neither simply the most active fish's solitary phenotype nor evidence that followers had surrendered all influence.[ref]
Social feedback and the emergence of leaders and followers by Jennifer L. Harcourt and others. 2009, individual assays, paired trials and movement-state model
A second route is division of labour based on developmental or physiological differences. Body size can alter the mechanical returns to defence or transport; age can alter experience, residual lifespan and the cost of risky work. Members can thereby specialize on tasks for which their relative performance is better, even if another individual performs more tasks better in absolute terms. However, morphology may also constrain a role rather than represent an adaptation specifically for the present task, and an age pattern alone does not identify its endocrine or social cause.
Honeybee experiments provide evidence for that distinction. Rearing workers in groups of different sizes and transplanting older bees into otherwise forager-deficient colonies altered endocrine and behavioural development. Young workers could begin foraging unusually early under changed colony conditions. These manipulations show that worker-worker interactions affect age polyethism; age is not an independent clock that irreversibly assigns each bee its task.[ref]
Honeybee colony integration: worker-worker interactions mediate hormonally regulated plasticity in division of labor by Z. Y. Huang and Gene E. Robinson. 1992, group-rearing and older-worker transplant experiments
Roles can be maintained through feedback without being individually optimal in every context. Repeated experience can improve information about a particular location, while repeated exclusion from reproduction can make helping the best available option. A dominance hierarchy can distribute access to food or breeding, but rank may reflect competitive constraints rather than efficient allocation. A subordinate's increased work may therefore result from limited alternatives or coercion, not from a freely chosen cooperative specialization. These possibilities predict different changes after removing dominant members or opening breeding opportunities.
At the group level, complementary tendencies can reduce duplicated effort, switching costs and interference. A mixture of initiators and responsive followers can exploit information that a uniformly cautious group would not use; different thresholds can spread effort across tasks. Yet too many risk-taking initiators may fragment a group, while excessive following may create dependence on poorly informed leaders. The effects therefore depend on composition, task demand and environmental variation. A positive association between behavioural diversity and performance is not enough to establish that selection maintains that diversity: group size, resource supply and group age may influence both.
Nor does specializing necessarily make a worker an expert. In Temnothorax albipennis, measurements across several tasks found that individual specialization did not predict higher task efficiency, and much work was not performed by the most efficient workers. This rejects a simple specialization-equals-skill explanation in that study. It leaves other possible benefits, including task coverage and reduced switching or coordination costs, to be tested independently.[ref]
Specialization Does Not Predict Individual Efficiency in an Ant by Anna Dornhaus. 2008, individual task performance and allocation of labour
Persistent differences can themselves be socially maintained. An individual repeatedly treated as a leader obtains more opportunities to lead; a member repeatedly excluded from one task acquires less experience in it. Social niche specialization can thus stabilize a distribution of roles through feedback between behaviour and partner responses. At the same time, phenotypic plasticity permits replacement after a worker or leader disappears. A group can display stable role proportions while its individual members change roles, so stability of organization should not be confused with rigidity of membership.
A causal study should follow identified individuals across repeated contexts, estimate behavioural repeatability after accounting for age and state, and measure partners' responses. Cross-fostering, standardized hunger manipulations, group-composition changes and member removals can distinguish pre-existing propensities from social induction. Performance should be measured separately from time allocated to a task, and group productivity separately from each member's reproductive success. These distinctions also expose cases in which a role benefits others while imposing costs on its occupant.
Consistent differences therefore supply biases from which social organization can emerge, but the resulting roles are conditional, relational and often reversible. The strongest explanation links an individual trait to a response rule, shows how interactions turn that rule into a role, and tests the consequences for both the individual and the group.
Relatedness is not required when responding to others yields a sufficient direct benefit, and coordination need not begin as costly altruism. Coordinated behaviour means that individuals adjust the timing, position or type of their actions relative to others. Cooperation concerns benefits provided through an interaction, while evolutionary altruism specifically imposes a direct fitness cost on the actor. Confusing these categories makes unrelated coordination appear harder to explain than it is.
Consider animals travelling together. Matching a neighbour's direction can reduce an individual's predation risk or help it reach food. Both the responder and the neighbour may benefit immediately; no deferred repayment or kin recognition is necessary. Likewise, complementary hunters can each increase their own chance of capture by responding to another's actions. The relevant condition is that the expected direct return to the response exceeds its costs, relative to available alternatives. That condition depends on ecology, not merely on whether companions share genes.
A clear interspecific example is joint hunting by groupers and giant moray eels, which cannot be close genetic relatives. Field observations documented nonrandom associations, grouper recruitment signals and benefits to both partners. Their different hunting modes expose prey that could evade either hunter alone. Each captured prey item is swallowed by its captor, limiting disputes over division of a carcass. The study supports a direct-benefit mechanism; it does not require alternating favours or prove that every recruitment signal evolved specifically in that association.[ref]
Interspecific communicative and coordinated hunting between groupers and giant moray eels in the Red Sea by Redouan Bshary and others. 2006, associations, recruitment and complementary hunting modes
Simple response rules can make individually advantageous actions fit together. Attraction, alignment, avoidance and following informed individuals can generate collective movement without central control. A quorum response makes commitment more likely after enough others act, potentially preventing one mistaken individual from drawing the whole group into danger. Such proximate rules still need an evolutionary explanation: heritable differences in responsiveness must affect expected survival or reproduction in the environments where the rule is expressed.
Experiments with three-spined sticklebacks used moving replica fish to manipulate apparent social information. Larger groups under perceived risk were less readily led by a single replica than solitary fish, and nonlinear response models explained these decisions better than simple proportional copying. Simulations linked these rules to improved decisions under specified assumptions. The experiment establishes a plausible coordination mechanism; actual lifetime fitness gains and the historical selection of its parameters remain separate questions.[ref]
Quorum decision-making facilitates information transfer in fish shoals by Ashley J. W. Ward and others. 2008, replica-fish experiments and decision models
The strategic problem also depends on the payoff matrix. In a coordination game, joining a hunt can be a best response when others join, while acting alone is better when nobody else participates. Shared cues, recruitment signals and learned conventions can move a group toward the mutually beneficial equilibrium. Here the difficulty is reaching or maintaining compatible choices. In a prisoner's dilemma, by contrast, withholding a contribution pays better against either partner action in a one-shot encounter. An account of coordinated hunting must establish which incentives actually apply rather than assume every group activity is a public-goods dilemma.
When cooperation does carry an immediate cost, direct reciprocity can make future consequences matter. In a deliberately simple repeated donation game, giving costs and benefits a partner by . If encounters continue with probability , perpetual mutual cooperation yields . Defecting once against a cooperator yields if it then triggers permanent noncooperation. Cooperation is preferable against that deviation whenThis is a conditional comparison under recognition, reliable observation and the specified retaliation rule. It is not a universal threshold for animal cooperation, nor does it show that a rare cooperative strategy can always invade an uncooperative population. Primary repeated-game modelling and computer tournaments established how such contingent interactions can sustain cooperation under suitable conditions.[ref]
The evolution of cooperation by Robert Axelrod and William D. Hamilton. 1981, theoretical model and strategy tournament
Other mechanisms need not involve repayment by the same individual. Partner choice can reward useful collaborators through access to future interactions; leaving an unproductive association can impose an opportunity cost on a defector. Reputation can alter future access to different partners. Partner fidelity feedback occurs when helping a partner increases the actor's future benefits because that partner survives or becomes more productive. These mechanisms require appropriate encounter structure, information and opportunities to choose; naming them is not evidence that a particular species uses them.
Evolutionary policing or partner sanctions can change the returns to exploitation. As a mechanistic example involving unrelated partners, soybean experiments prevented a normally fixing rhizobial strain from fixing nitrogen by changing its atmospheric supply. Reduced bacterial reproductive success and oxygen-supply measurements supported a host-sanction interpretation. This shows how conditional resource allocation can favour service provision without kinship, although it is not by itself an example of synchronized animal movement or proof of the historical origin of the interaction.[ref]
Host sanctions and the legume-rhizobium mutualism by E. Toby Kiers and others. 2003, experimental prevention of nitrogen fixation and symbiont performance
Coordination can consequently evolve through several routes: immediate mutual benefit, stable contingent exchange, partner assortment, or changed incentives imposed by others. Learning can implement or transmit successful rules, while genetic evolution shapes learning capacities and costs. These explanations are compatible with multilevel descriptions of selection, but a claim that groups benefit is insufficient unless the process maintaining the relevant individual strategies is specified. Effective groups of unrelated individuals emerge when responding and contributing are viable strategies in their actual ecological and social setting.
Dependence evolves when a partner becomes a sufficiently reliable part of the environment that specialization on its services outcompetes maintaining an autonomous alternative. Reciprocal evolutionary change requires additional evidence. Ecological interdependence, obligate symbiosis and coevolution describe different properties: present-day benefit, inability to persist without assistance, and reciprocal heritable responses to selection, respectively.
An association can begin with incidental benefits. One species releases metabolic products, modifies habitat or consumes a toxin; another uses the altered environment. Initially neither partner need have evolved a service for the other. Repeated association can favour increased access to that benefit, spatial attachment or mechanisms that exchange complementary resources. Metabolic cross-feeding may arise from waste uptake before either producer becomes dependent on a particular recipient. This route requires no foresight and does not imply that the interaction started as costly altruism.
Once a service is sufficiently reliable, retaining an expensive redundant function may yield little advantage. Adaptive gene loss can then make the recipient dependent. Neutral deterioration under relaxed selection is another possible route, particularly when small populations and transmission bottlenecks weaken purifying selection. These explanations have different predictions about costs and selection and should not be conflated: a missing gene is not evidence, by itself, that losing it was adaptive. Moreover, dependence is conditional on the environment. A lineage unable to grow alone in one natural setting may grow without its usual partner when the missing resource or protection is experimentally supplied.
Experiments with Prochlorococcus illustrate this distinction. The cyanobacterium is vulnerable to extracellular hydrogen peroxide, and co-culture with peroxide-removing Alteromonas protected cells and enabled growth at low densities. Removing the surrounding microbial community also altered peroxide accumulation in seawater assays. These results establish an ecological dependence on a diffusible protective service in the tested conditions. They do not demonstrate that one specific helper species must be present, that helpers require Prochlorococcus in return, or that gene loss and reciprocal adaptation were observed evolving during the experiment.[ref]
Dependence of the Cyanobacterium Prochlorococcus on Hydrogen Peroxide Scavenging Microbes for Growth at the Ocean's Surface by J. Jeffrey Morris and others. 2011, peroxide measurements, co-culture and growth experiments
Reciprocal specialization can make dependence bilateral. If each partner increasingly relies on a different product or function supplied by the other, selection can favour complementary investment and reduced redundancy. Inherited association strengthens that feedback: successful host reproduction also transmits symbionts, so investment in host function can improve symbiont transmission. Vertical transmission and physical compartmentalization can therefore align some fitness consequences. They do not make interests identical, because symbionts can still compete within hosts and hosts can favour reduced costs of support.
Aphids and Buchnera aphidicola provide a strong example of a highly integrated association. The sequenced Buchnera aphidicola genome has extensive losses but retains pathways associated with essential amino-acid provision, consistent with nutritional complementation of the aphid's diet. The bacterium depends on the host-associated setting, while the host uses its biosynthetic contributions. This pattern supports derived specialization and loss of autonomy; the genome alone does not establish every metabolite exchanged or directly reconstruct the order of historical evolutionary changes.[ref]
Genome sequence of the endocellular bacterial symbiont of aphids Buchnera sp. APS by Shuji Shigenobu and others. 2000, reduced genome and retained biosynthetic functions
Dependence can also arise through repeated behavioural or ecological specialization rather than physical integration. A pollinator can specialize on a floral resource, or a predator on a particular prey. The affected partner may then evolve recognition, defence or counter-exploitation. Such interactions may remain facultative, asymmetric or antagonistic. Conversely, obligate association can arise through one lineage's losses while the other changes little. Thus the intensity of current dependence does not measure the amount of reciprocal evolution.
Coevolution requires each lineage to alter selection on the other, with a heritable response in both. A functional match between two traits is insufficient: both could have adapted to the same abiotic environment, one could have tracked the other, or different partners could produce the same match. An association might also result from ecological sorting of already compatible types. Immediate behavioural adjustment or altered gene expression is phenotypic plasticity unless an inherited change in the response itself is demonstrated.
Experimental host-parasite evolution gives a clearer test. In replicated populations of bacteria and bacteriophages, temporal comparisons of bacterial resistance and phage infectivity demonstrated reciprocal escalation, with divergence among replicate populations. Here changes in the antagonist's traits change the selective environment confronting the other lineage. This is evidence for an antagonistic arms race rather than merely a close ecological association. It also shows why coevolution is not restricted to beneficial partnerships.[ref]
Antagonistic coevolution between a bacterium and a bacteriophage by Angus Buckling and Paul B. Rainey. 2002, experimental resistance-infectivity dynamics and between-population differentiation
For a mutualism, reciprocal-transplant experiments can cross evolved hosts with ancestral and evolved symbionts, measuring both parties' performance in a common environment. Parallel evolution without the partner and controls for adaptation to the culture medium help isolate partner-mediated selection. In natural systems, time-shift assays, reciprocal genotype combinations and evidence that relevant traits affect partner fitness strengthen an inference; simple correlations and matching phylogenies remain vulnerable to shared environmental or transmission histories. Diffuse coevolution involving several interchangeable partners is possible and need not produce a one-to-one species pair.
The result may be complementary specialization and increasingly integrated reproduction, but stability is not guaranteed. Cheaters, changing environments, loss of partners and altered transmission can destabilize even an obligate association. The transition from incidental benefit to dependence is therefore explained by the relative costs of autonomy and association; the transition to coevolution is established only when reciprocal selection and heritable responses are demonstrated.
Conflicts are reduced by changing who benefits from cooperation, constraining opportunities for selfish success, or imposing costs on exploiters. The same logic operates between organisms and inside them, but the units that reproduce and transmit differ. Resolution need not mean eliminating all conflict or giving every participant its preferred outcome: it can be a stable compromise, suppression by a powerful party, or a continuing arms race.
An evolutionary conflict exists when different inherited strategies or replicating lineages favour different outcomes. Between organisms, individuals may disagree over resources, mating or contributions to a shared activity. Within an organism, cell lineages can gain from proliferating at their neighbours' expense, and genes can gain a transmission advantage that harms the rest of the genome. A common environment or membership of one body does not guarantee identical interests.
Between organisms, alignment can make restraint individually worthwhile. Genetic relatedness can reward benefits to relatives through inclusive fitness; repeated interaction can link current help to later returns; and partner choice can make productive cooperation a condition of continued association. Reliable exchange can also make a partner's survival directly valuable. None of these mechanisms requires conscious agreement. They work only where their gains outweigh the available selfish alternative, including the costs of assessment and enforcement.
Conditional allocation supplies another route. In soybean experiments, preventing rhizobial nitrogen fixation reduced bacterial reproductive success, while physiological measurements implicated reduced oxygen supply to non-fixing nodules. This supports host control that makes poor service costly to the symbiont. The treatment forced noncooperation in an otherwise cooperative strain: it tests the consequences of service failure, rather than demonstrating the evolutionary origin of a particular cheating mutation.[ref]
Host sanctions and the legume-rhizobium mutualism by E. Toby Kiers and others. 2003, nitrogen-free atmosphere treatment and nodule responses
Social insects show how relatedness and enforcement interact without making a colony conflict free. Workers can produce haploid sons, creating disagreement over male production. With a sufficiently multiply mated queen, a worker may be more related to queen-produced males than to the average other worker's sons. Experiments in honeybees found strong discrimination against worker-laid male eggs, supporting worker policing. The result establishes differential treatment of eggs; relatedness and colony productivity are possible selective benefits and must be evaluated rather than assumed equivalent.[ref]
Worker policing in the honeybee by Francis L. W. Ratnieks and P. Kirk Visscher. 1989, genetic incentives and experimental egg discrimination
Within multicellular organisms, common descent changes the baseline. Development from a single-cell bottleneck normally makes most cells close genetic relatives and links their lineage's long-term transmission to successful reproduction of the organism. Germline-soma differentiation further restricts the routes by which a proliferating somatic lineage can reach future generations. These features help explain extensive cellular cooperation, but they are incomplete protection: somatic mutation can create a clone that grows faster within the body even while lowering host survival or reproduction.
Cell-cycle regulation, DNA-damage responses, apoptosis, tissue architecture and immune responses can restrict such expansion. Some mechanisms remove damaged cells; others reduce opportunities for spread or prevent extra divisions from translating into transmission. Their developmental and maintenance functions mean that they should not all be described as adaptations exclusively for cancer suppression. Cancer demonstrates that the constraints can fail, especially when selection on the organism is weak at ages after most reproduction.
Apoptosis and cell competition are also not automatically measures of collective welfare. In experimental Drosophila tissues, higher Myc expression made clones eliminate lower-Myc neighbours and expand at their expense. This showed that a process involving elimination of neighbouring cells can be exploited by a locally successful lineage. It cautions against labelling whichever cells win a contest “best for the organism.”[ref]
dMyc Transforms Cells into Super-Competitors by Eduardo Moreno and Konrad Basler. 2004, mosaic tissues, neighbour elimination and clonal expansion
Genetic conflict can persist even when cells descend from one zygote, because loci may have different transmission rules. A sex-linked meiotic driver can increase its own representation by impairing gametes carrying the alternative chromosome. Autosomal alleles can instead favour restoration of a more balanced transmission system. In Drosophila simulans, genetic and molecular work identified the autosomal suppressor not much yang, which suppresses an X-linked sex-ratio distorter; cytological work connected distortion to failure of Y-bearing sperm maturation. This is a concrete case of a genomic countermeasure, rather than an assumption that Mendelian inheritance is intrinsically immune to selfish elements.[ref]
A sex-ratio Meiotic Drive System in Drosophila simulans. I: An Autosomal Suppressor by Yun Tao and others. 2007, suppressor characterization and sperm-development evidence
The comparison reveals two common principles. First, common transmission can align interests, as in relatives, vertically transmitted symbionts and clonally developing cells. Second, discrimination can make selfish strategies less profitable, as in partner sanctions, worker egg removal and suppression of a driver. Compartmentalization can help target the responsible partner or lineage, but its effect depends on scale: a compartment founded by one symbiont may reduce within-compartment mixing while still allowing competition among host compartments.
There are also important differences. Separate organisms can often leave, switch partners or use outside resources, so the costs of exit shape bargaining and partner choice. An ordinary somatic cell has few such reproductive alternatives and is usually integrated into a developmentally specified body. Genes inside that cell cannot choose partners in the behavioural sense, but recombination, linkage and differential transmission change the selection acting on suppressors. At either scale, suppression can select for evasion, producing continuing counteradaptation rather than permanent harmony.
A successful explanation therefore specifies the competing units, their routes of transmission, the benefit of the proposed control mechanism, and the level at which success is measured. More offspring, more surviving symbionts, a larger clone and greater representation of one chromosome are different outcomes. Conflicts are resolved to the extent that mechanisms make the lower-level selfish alternative less successful relative to its competitors; neither organismal organization nor social cooperation is evidence that the underlying conflict has vanished.
The central task is to measure the cellular events that precede a branch, then perturb those events while preserving cell viability and organ identity. Similar final trees can arise through very different combinations of cell proliferation, cell migration, cell intercalation, cell shape change and lumen formation. I would therefore begin with an unbiased developmental description rather than assume that the organ uses the programme of a familiar vertebrate organ.
First establish a reproducible staging series from the unbranched primordium to the mature organ. Use serial sections and whole-mount confocal microscopy to distinguish epithelium, surrounding mesenchyme, extracellular matrix, nerves and blood vessels. Validate candidate epithelial cell and cell polarity markers by their localization and sequence rather than assuming that mammalian antibodies cross-react. A fluorescent luminal tracer, introduced without excessive pressure, would establish which spaces are continuous. Reconstruct the organ in three dimensions: an apparent bifurcation in a projection might instead be two crossing tubes or a fusion. Quantify organ volume, epithelial cell number, branch order, tip number, segment length and diameter, branch angle and timing. Distinguish lateral budding, tip bifurcation and branch fusion. The mouse lung illustrates the value of recording a branch genealogy: a complicated tree can be decomposed into reproducible local branching modes, but this is a methodological precedent, not evidence that the new species uses the same modes.[ref]
The branching programme of mouse lung development by Ross J. Metzger and others. Developmental reconstruction and identification of local branching modes
Next establish intact-animal live-cell imaging, preferably with light-sheet fluorescence microscopy if optical access allows it, and a complementary explant culture containing both epithelium and mesenchyme. Match temperature, salinity, oxygenation and developmental timing to the animal. Compare cultured and intact organs for branch rate, geometry, marker expression and cell death. Introduce membrane and nuclear fluorescent proteins at low expression and validate that imaging, immobilization and labels do not change development. Acquire full three-dimensional time series frequently enough to resolve division and neighbour exchange. Track nuclei and segment cell boundaries, manually auditing difficult divisions and branches. Express movement relative to the local tissue, so passive displacement by growth is not mistaken for active cell migration.
Measure separately the sources of tissue expansion. Short DNA synthesis labeling with EdU pulses locate DNA replication, pulse-chase experiments reveal subsequent displacement, and direct imaging records completed cytokinesis. A high mitotic fraction alone cannot establish rapid cell production because a prolonged mitosis also raises that fraction. Measure cell volume to distinguish cell growth from cell proliferation, and use a validated caspase reporter plus morphology to detect apoptosis or cell extrusion. For an explicitly bounded region, the bookkeeping identity is , where counts completed divisions in the region, deaths and live-cell entries and exits across its boundary. This checks whether tracked behaviours explain the measured cell-number change; lumen inflation or stretching can enlarge the organ without increasing .
Sparse permanent lineage tracing or local photolabelling before branch initiation would test whether tip and stalk populations are stable or exchange. Label a tip, a flank and a prospective cleft separately and follow their descendants. Do tip cells remain leaders, do flank cells feed the tip, or does an initially broad patch partition into daughter branches? Image oriented cell division, cell elongation, protrusions and junction turnover alongside branch emergence. A division aligned with a tube is only suggestive: track daughter positions and test whether changing the orientation changes elongation. Quantify neighbour exchanges to identify cell intercalation. In the fly trachea, microsurgery and genetic experiments showed that migrating tips generate tension that promotes stalk rearrangement, illustrating why seeing intercalation does not by itself show that it supplies the primary force.[ref]
Tip-cell migration controls stalk-cell intercalation during Drosophila tracheal tube elongation by Emmanuel Caussinus and others. Genetic and microsurgical tests of tip-generated tension
Then make acute, staged causal tests. Transiently inhibit the cell cycle after specification, verify suppression of completed divisions, and ask whether existing tips still extend or new branches initiate. Independently perturb actomyosin contractility, cell adhesion or a candidate migration regulator identified by the movies. Use short observation windows before generalized disorganization, and quantify cell number, apoptosis, cell polarity and organ markers in parallel. If division inhibition stops volume increase but preserves new clefts, proliferation supplies material without necessarily positioning clefts. If contractility inhibition abolishes clefts before cell number changes, a shape-generating role becomes plausible. Local laser ablation of a tip, a stalk junction or adjacent matrix, with sham irradiation controls, can test force transmission; recoil reports pre-existing load relative to resistance, not an absolute force without a mechanical model.
Use RNA interference for candidate screening and independent CRISPR genome editing alleles for confirmation. Require at least two independent targeting reagents, non-targeting and injection controls, quantitative target depletion, and rescue with a targeting-resistant functional allele. Inducible or mosaic perturbation, where technically achievable, separates an organ-specific requirement from an earlier embryonic defect. Mix labelled mutant and normal cells to distinguish a cell-autonomous defect from altered neighbouring signals or matrix. Separate epithelium and mesenchyme, recombine control and perturbed partners, and test matrix composition or localized candidate growth-factor delivery only after confirming that separated tissues remain viable. Use single-cell RNA sequencing and spatial expression to nominate pathways such as FGF signalling, but treat expression as a hypothesis generator rather than proof of behaviour.
Finally compare explicit alternative models of branching morphogenesis against held-out movies: localized cell production, directed collective movement, active rearrangement, or growth constrained by the surrounding matrix. Each should predict both branch geometry and the observed cell trajectories, and its response to a spatially restricted perturbation. Randomize treatment, blind segmentation and use animals from independent clutches as biological replicates; many cells within one animal do not replace independent animals. The strongest outcome is a causal chain from molecular perturbation to altered cell behaviour to altered branch geometry, supported by rescue and by measurements showing that general developmental delay cannot explain it.
Intestinal development constructs a patterned renewing organ; intestinal homeostasis continually replaces its cells while preserving that organization. Both depend on reciprocal signalling between endoderm-derived epithelium and mesenchyme, but they solve different problems. Development expands and regionalizes the tissue, establishes architecture and produces its first mature cell types. Adult tissue homeostasis balances cell production, cell differentiation, movement and loss within an already established architecture. The mammalian small intestine provides the main comparison; its villi and crypts should not be indiscriminately attributed to the colon or to all vertebrates.
Early intestinal development begins with a broadly proliferative epithelial tube whose regional identity is established in its embryonic context. Factors including CDX2 help impose intestinal identity, while local signals distinguish the future small intestine and colon. Growth is coordinated with the formation of smooth muscle, connective tissue, the enteric nervous system and vasculature. The emergence of intestinal villi transforms a relatively simple luminal surface into an absorptive one. In mouse, epithelial Hedgehog signalling promotes underlying mesenchymal clusters, and BMP signalling helps space those clusters. In explants, increased BMP activity suppresses clusters whereas BMP inhibition produces merged clusters and abnormal villus patterns. This supports a role in pattern generation, not simply in the terminal differentiation of enterocytes.[ref]
Villification in the mouse: Bmp signals control intestinal villus patterning by Katherine D. Walton and others. Explant BMP perturbations and the comparison with chick villification
The mechanics and signalling must be distinguished across species. In chick, sequential smooth muscle differentiation constrains growth, generating ridges, zigzags and villi through buckling. In mouse, patterned mesenchymal clusters arise before equivalent surface deformation, so the chick sequence is not a general account of mammalian villus initiation. The common principle is reciprocal communication between layers; the ordering of mechanical and chemical patterning differs. In development, therefore, an abnormal villus pattern could arise from defective mesenchymal organization, epithelial growth or mechanical coupling, even if the final epithelial cell differentiation markers are present.
As villi emerge, proliferative cells become concentrated in intervillus regions, and intestinal crypts develop chiefly around the perinatal and postnatal transition in mouse. The fetal proliferative epithelium is consequently not simply a miniature adult crypt. Paneth cells and other components of the mature niche also appear on their own developmental schedules. Demonstrating an adult stem-cell marker in an embryonic cell would not alone establish that the embryonic lineage hierarchy or niche requirements are identical to the adult ones.
In adult small-intestinal tissue homeostasis, cycling Lgr5 positive intestinal stem cells at crypt bases generate renewed stem cells and transit-amplifying cells. Descendants differentiate into absorptive enterocytes and secretory populations including goblet cells, enteroendocrine cells, tuft cells and Paneth cells. Most differentiated descendants move toward the villus tip and are shed, whereas Paneth cells occupy the crypt base. lineage tracing from the Lgr5 locus generated persistent contributions to all epithelial lineages, providing functional evidence for self-renewal and multipotency rather than relying on marker expression alone.[ref]
Identification of stem cells in small intestine and colon by marker gene Lgr5 by Nick Barker and others. Inducible lineage tracing and persistence of labelled epithelial lineages
The adult niche spatially restricts developmental pathways. High local Wnt signalling and R-spondin support crypt stemness and growth, while BMP signalling restrains crypt-like programmes outside their appropriate domain. Notch signalling favours absorptive over secretory lineage allocation partly by opposing ATOH1-dependent secretory specification. Thus a single pathway can control both population maintenance and cell composition: stimulating proliferation is not sufficient if the resulting cell differentiation balance is wrong. Stromal signals are essential in vivo, and Paneth cells provide additional local support in small intestine; the colon maintains stem cells without a small-intestinal Paneth-cell arrangement. Niche dependence cannot therefore be equated with dependence on one invariant supporting cell type.
The adult organ is dynamically stable rather than cellularly static. A stem-cell clone can expand while neighbouring stem-cell clones disappear through neutral drift, with the total compartment maintained.[ref]
Intestinal crypt homeostasis results from neutral competition between symmetrically dividing Lgr5 stem cells by Hugo J. Snippert and others. Multicolour clonal tracing and neutral-drift analysis
At the organ level, sustained excess production generates expansion or neoplasia; excess loss causes barrier failure. Development deliberately changes total cell number, surface area and proportions over time, whereas adult maintenance constrains their long-term averages. Nevertheless, adult tissue homeostasis remains responsive to feeding, microbes, immune signals and injury, and is not a completely fixed endpoint.Experimental models expose both continuity and differences. A single sorted Lgr5 positive cell can produce a self-renewing intestinal organoid containing organized differentiated progeny in a suitable matrix and supplied growth factors. This establishes epithelial self-organization under defined conditions, not niche independence in the absence of extracellular signals: the medium replaces important niche functions.[ref]
Single Lgr5 stem cells build crypt-villus structures in vitro without a mesenchymal niche by Toshiro Sato and others. Single-cell cultures, lineage organization and defined culture requirements
Embryonic explants retain the mesenchyme needed to study villus patterning, while adult intestinal organoids are especially useful for stem-cell maintenance and lineage allocation. Neither alone reproduces an intact organ's circulation, innervation, immune environment and longitudinal regionalization.Finally, injury reveals an important bridge between development and maintenance. cell fate plasticity can restore missing stem cells, so the normal adult lineage flow is not an irreversible restriction of all descendants. Committed progenitor cells can recover stem-cell function under particular injury conditions, but this does not establish that all mature villus cells routinely do so. A decisive comparison uses stage-specific lineage tracing, matched marker analysis and timed pathway perturbation, measuring architecture and functional output as well as cell proliferation. Development and adult renewal reuse molecular machinery while differing in tissue geometry, developmental competence and the direction of net population change.
Epithelial cell fate plasticity is a context-dependent change in developmental potential or differentiated identity. It includes dedifferentiation toward a progenitor cell state, transdifferentiation between differentiated identities, and reversible intermediate states. It is distinct from selecting a pre-existing rare stem cell, and from ordinary progression down a lineage. epithelial-mesenchymal plasticity is one important form, but changing epithelial subtype without losing epithelial organization is also cell fate plasticity.
The strongest physiological rationale is that a tissue needs both stable specialization and reserve routes for replacement. During ordinary adult tissue homeostasis, a stem-cell hierarchy can efficiently supply predictable cell types. After injury removes a component of that hierarchy, local signals and newly available stem-cell niche space may permit a committed descendant to reacquire self-renewal. In mouse intestine, Alpi marked enterocyte-lineage progenitor cells normally generate short-lived absorptive descendants. After targeted ablation of Lgr5 positive intestinal stem cells, labelled progenitor cells can generate long-lived crypt-villus lineages with renewed stem-cell output. Comparing the same labelled population before and after ablation distinguishes injury-dependent cell fate plasticity from its normal fate. The experiment concerns progenitor cells in the enterocyte lineage; it should not be generalized to every terminally mature villus enterocyte.[ref]
A complementary model is the mouse airway. Genetic depletion of basal stem cells, combined with prior lineage tracing of luminal secretory cells, revealed secretory-cell descendants that acquired basal-cell properties and sustained subsequent epithelial production. Experiments with isolated cells and cocultures further showed that contact with basal cells inhibits this conversion. cell fate plasticity is therefore regulated by the tissue environment, not simply an intrinsic capacity unmasked whenever a marker changes. Its interpretation requires controls for residual basal cells and for whether the secretory-lineage driver labelled basal cells before injury.[ref]
Dedifferentiation of committed epithelial cells into stem cells in vivo by Purushothama Rao Tata and others. Basal-cell ablation, secretory-cell lineage tracing and contact-dependent suppression
Development provides additional contexts. Embryonic epithelia can undergo epithelial-to-mesenchymal transition during processes such as gastrulation, and mesenchymal-to-epithelial transition can subsequently assemble epithelial structures. These are regulated changes in adhesion, cell polarity, motility and gene expression, rather than a simple binary switch read from E-cadherin alone. In wound repair, transient relaxation of epithelial organization can facilitate migration while retaining intercellular contacts. A partially migratory repair state need not entail a complete mesenchymal conversion or a permanent change of lineage. Following wound closure, restoration of barrier function and polarized architecture is as important as the initial ability to move.
The most convincing experimental design labels a defined starting population irreversibly before the inducing event, allows the inducer to clear, then follows labelled descendants through the transition. Check immediate labelling specificity, include no-inducer and uninjured controls, quantify labelling efficiency and rule out ectopic driver activation after injury. Demonstrate the new state with multiple markers, morphology and function, and persistence after the inducing signal is removed. Serial epithelial production or a second injury challenge tests stable self-renewal; a transient appearance of a basal marker does not. Sparse labelling and continuous live-cell imaging help distinguish conversion from contamination, cell fusion or selective expansion of a rare initially unrecognized progenitor cell.
single-cell RNA sequencing can identify intermediate cell states and candidate regulators, but inferred trajectories are not lineage histories. Combine it with genetic barcodes, spatial localization and timed perturbation of candidate transcription factors or niche signals. Organoids offer defined media, prospective cell isolation and manipulation of matrix stiffness. A sorted population's ability to make a structure in culture establishes potential under those conditions; dissociation and a permissive medium may induce a capacity rarely used in vivo. Compare culture results with intact-tissue fate mapping before claiming a normal physiological contribution.
The evolutionary argument is a trade-off, rather than a claim that every plastic response is an adaptation. Conditional access to alternative cell fates could buffer environmental injury and permit repair without maintaining a separate reserve stem-cell pool for every possible lesion. Conserved signalling modules can also be redeployed in new developmental contexts. These advantages must be weighed against loss of specialized function, energetic costs and the danger of inappropriate persistent growth. Comparative experiments should ask whether homologous lineages undergo similar transitions under comparable injuries; shared expression of a few regulators is insufficient to prove that an ancestral cell fate plasticity programme has been conserved. At the tissue level, cell fate plasticity supplies alternative states on which selection can act, but it does not itself establish heritable evolutionary change.
Clinically, controlled cell fate plasticity may improve epithelial repair, provide transplantable cells and make patient-derived disease models. The same capacity can undermine treatment: a tumour may switch to a less drug-sensitive lineage or regenerate a stem-like population after therapy. In carcinoma, epithelial-mesenchymal plasticity can contribute to invasion and treatment resistance, but neither a single EMT marker nor its absence establishes the mechanism of metastasis. In a lineage-traced mouse lung-cancer model, the tested EMT programme was dispensable for lung metastasis while contributing to chemoresistance; the conclusion is specific to that model and reporter coverage.[ref]
Epithelial-to-mesenchymal transition is not required for lung metastasis but contributes to chemoresistance by Kari R. Fischer and others. Lineage-tracing and chemotherapy experiments in mouse tumours
The useful clinical aim is therefore a defined, reversible transition that restores function, with evidence that it does not leave a persistently proliferative or malignant population.reactive oxygen species can alter competitive fitness, but neither high ROS nor an antioxidant response universally identifies a loser. cell competition is relative: cells that survive in one neighbourhood are preferentially lost in another, with fitter neighbours occupying their place. An experiment showing oxidant-induced death in a homogeneous tissue establishes toxicity, not necessarily cell competition. In epithelia, loss can occur through apoptosis, extrusion or differentiation followed by departure from a proliferative layer.
reactive oxygen species include superoxide and hydrogen peroxide, which differ in reactivity, localization and transport. They can arise from mitochondrial metabolism or regulated oxidase activity. At controlled levels they participate in redox signalling; excess or poorly buffered production damages DNA, proteins and membranes. Competitive fitness can therefore change through altered damage, stress responses, growth or differentiation. NRF2 and its fly counterpart CncC regulate antioxidant and detoxification programmes. Their activation is an integrated response to cellular conditions, not a direct quantitative measurement of one ROS species.
An instructive fly study compared prospective losers carrying a ribosomal-protein defect or loss of Mahjong protein. Both activated antioxidant-response genes before elimination. In ribosomal-protein-deficient cells, two ROS dyes did not reveal a uniform increase, whereas reduced-thiol staining was lower. Mild CncC activation was tolerated across an entire disc but caused boundary-enriched death in clones surrounded by normal cells; those clones survived better among less-fit neighbours. Conversely, reducing CncC impaired stressed-cell survival. Thus a protective response can also confer relative loser status. The study separated this module from JNK signalling effects on growth and from JAK-STAT signalling effects on tissue expansion; it did not establish a compulsory linear chain from ROS through JNK to elimination.[ref]
Chronic activation of JNK JAK/STAT and oxidative stress signalling causes the loser cell status by Iwo Kucinski and others. Figures 5–7, redox measurements and neighbourhood-dependent CncC experiments
This distinction prevents two errors. First, a high antioxidant-response reporter can coexist with successful buffering and relatively low measured oxidant levels. Second, knocking down a protective factor may kill cells autonomously, making their apparent competitive loss worse even if that factor also participates in neighbour-dependent recognition. To identify a competitive mechanism, compare the same genotype in a homogeneous tissue, in a mosaic with normal neighbours and in a mosaic with an alternative neighbour genotype. Quantify clone growth, death at boundaries and in centres, and replacement by neighbours, normalized to the corresponding cell numbers or areas. A clone that is small because its cells divide slowly has not necessarily been actively eliminated.
The adult mammalian oesophagus supplies a striking environmental example. In transgenic mouse epithelium, low-dose ionizing radiation induced an oxidative response that shifted normal basal cells toward differentiation. Cells carrying mutant p53 were relatively insensitive and expanded at their neighbours' expense. Combining antioxidant treatment with irradiation reversed the population outcome, promoting normal-cell proliferation and mutant-cell differentiation. The selective advantage was consequently conditional on the redox environment, not a fixed property of the mutation. This also shows that competitive replacement need not be executed primarily by apoptosis.[ref]
A separate mouse experiment generated a mosaic of NRF2-deficient and NRF2-intact oesophageal cells. Deficient cells persisted under unstressed conditions but accumulated damage and were preferentially lost during exposure to the carcinogen 4-nitroquinoline 1-oxide. Tumours predominantly arose from the surviving NRF2-intact population. This supports a context-dependent role for stress protection in population selection, while not proving that every disappearing cell was directly recognized and killed by a neighbour. Carcinogen detoxification and DNA damage are additional variables, so the experiment is not a chemically pure ROS titration.[ref]
Cellular Nrf2 Levels Determine Cell Fate during Chemical Carcinogenesis in Esophageal Epithelium by Makoto Horiuchi and others. Mosaic deletion, unstressed controls and 4NQO exposure experiments
To test a proposed ROS mechanism in an epithelial mosaic, image a calibrated, compartment-targeted redox biosensor before clone loss, along with cell boundaries, a proliferation readout and a death or differentiation reporter. Include sensor controls for pH, expression level and dynamic range; general oxidant dyes have loading, localization and chemical-specificity limitations. Perturb the source and scavenging machinery independently and restrict the perturbation to prospective losers or winners. For example, a validated catalase manipulation tests peroxide buffering, while a source-specific perturbation tests whether that peroxide is required. A matched rescue should restore both the measured redox change and the competitive outcome. Monitor cellular energy and survival in homogeneous controls because a mitochondrial perturbation can affect fitness independently of ROS. Perturb downstream stress signalling separately to distinguish oxidant production, stress detection and execution of cell loss.
The tissue consequences can be beneficial or harmful. Elimination of damaged cells can preserve a barrier, but a stress-resistant mutant can also exploit environmental oxidants to displace normal cells. Persistent stress signals from damaged or dying cells may alter neighbour proliferation and inflammation, producing further changes in fitness. The experimentally supported conclusion is that redox state reshapes the conditions under which cells persist, differentiate or are eliminated. A universal prescription to raise ROS or administer antioxidants does not follow: the relevant species, tissue compartment, neighbour genotype and exposure history determine the direction of selection.
positional information allows cells to choose an appropriate developmental response for their location; positional memory allows a location-dependent identity to persist after the original signal has changed. Neither is identical to cell differentiation. Two connective-tissue cells can have similar current functions but different information about where they belong in a limb. Development must establish these relationships, while regeneration must reconstruct missing relationships from an incomplete stump.
In the classical positional information framework, a tissue first establishes coordinates and cells interpret them according to their competence and developmental history. A morphogen gradient is one possible coordinate system. Different thresholds can elicit different gene expression states, but concentration alone is not the entire signal: exposure duration, feedback, changing tissue geometry and the response network also matter. Thus the same positional signal can produce different differentiated structures in different competent tissues.[ref]
Positional information and the spatial pattern of cellular differentiation by Lewis Wolpert. The separation of positional specification from cellular interpretation
The vertebrate limb bud is patterned along three interacting axes: proximal-distal, anterior-posterior and dorsal-ventral. The apical ectodermal ridge supplies FGF signalling that supports distal outgrowth and survival. Its early removal causes distal truncation, but this does not uniquely demonstrate that cells measure time in a progress zone: cell loss, altered growth and loss of signals can also change the structures that remain.[ref]
Positional Information in Chick Limb Morphogenesis by Dennis Summerbell and others. Classical progress-zone formulation and limb-bud experiments
Distal FGF signals and proximal influences interact with Hox genes and other regulators to organize stylopod, zeugopod and autopod territories. One must distinguish a positional identity defect from a failure to supply enough cells to execute that identity.Anterior-posterior patterning provides a more direct signal-relocation test. Grafting posterior zone of polarizing activity tissue to the anterior of a chick limb bud produces duplicated digit patterns. Sonic hedgehog is expressed in the posterior region, and anterior implantation of cells expressing it reproduces polarizing activity. This connects a localized molecular signal to a change in spatial identity, rather than merely correlating expression with posterior development. Digit pattern still depends on signal duration, growth and downstream regulation; a static concentration-to-digit lookup table is inadequate.[ref]
Sonic hedgehog mediates the polarizing activity of the ZPA by Robert D. Riddle and others. Expression analysis and anterior implantation of SHH-expressing cells
Along the dorsal-ventral axis, dorsal Wnt7a promotes Lmx1b in mesenchyme, while ventral Engrailed-1 helps restrict dorsal signalling. Interactions among these systems allow outgrowth and coordinate specification to remain aligned.Regeneration adds the problem of interpreting an amputation plane. An axolotl limb usually replaces structures distal to the cut: a wrist-level stump does not routinely add a new upper arm before rebuilding the hand. This implies that regenerative outgrowth retains or reconstructs level-specific information. A blastema contains proliferative progenitor cells beneath a specialized wound epithelium, but it is not a uniformly pluripotent mass. Transgenic graft and lineage experiments showed substantial memory of tissue origin and differences among progenitor cell populations. The distinction between tissue identity and spatial identity is essential: producing cartilage does not alone show that its proximal-distal address is correct.[ref]
Cells keep a memory of their tissue origin during axolotl limb regeneration by Martin Kragl and others. Labelled tissue grafts and lineage-restricted contributions to the blastema
Retinoid experiments show that positional identity can be reprogrammed. Treatment of distal axolotl amputations with vitamin A or related retinoids can generate proximal structures before distal ones, sometimes producing a much more complete limb from a distal stump. This is difficult to explain as simple acceleration of growth, because the identities and sequence of regenerated structures change. It supports proximalization of the responding tissue. Nevertheless, pharmacological reprogramming does not by itself prove that an endogenous retinoid gradient is the sole normal coordinate system; dose-dependent toxicity and effects on growth must be assessed separately.[ref]
Vitamin A and pattern formation in the regenerating limb by Malcolm Maden. Proximal-distal duplications after retinoid treatment of axolotl amputations
Spatial confrontation supplies another test. In an accessory-limb assay, a wound with appropriate nerve support can be combined with tissue of a different circumferential identity. Productive anterior-posterior interactions can support a patterned extra outgrowth, whereas wound healing and proliferation alone need not generate a complete limb. In axolotl experiments, anterior FGF8 and posterior Sonic hedgehog activities were identified as interacting signals, and manipulating them could replace aspects of the normally required tissue confrontation. This connects positional disparity to a signalling circuit that promotes regeneration, without implying that FGF8 and SHH encode every spatial identity by themselves.[ref]
FGF8 and SHH substitute for anterior–posterior tissue interactions to induce limb regeneration by Eugen Nacu and others. Signal localization and substitution in regenerative assays
A rigorous molecular test would transplant permanently labelled connective-tissue cells between defined limb positions, score their contribution and spatial identity, and perturb a candidate positional regulator specifically in those cells. Compare position-matched grafts, rotated or mismatched grafts, sham operations and equal nerve support; measure survival and proliferation so that graft failure is not mistaken for lost positional identity. Assess skeletal pattern and lineage output as well as positional markers, with rescue of the candidate perturbation. Such experiments separate a stable address, responsiveness to local signals and a generic requirement for outgrowth. Development and regeneration reuse signalling pathways, but regeneration additionally depends on retained information, wound-specific competence and communication between cells carrying different positional histories.
The developing mammalian heart grows by a changing combination of progenitor cell recruitment and division of differentiated cardiomyocytes. Differentiation is therefore not synonymous with permanent cell-cycle exit. Premature differentiation can exhaust a progenitor cell pool, while delayed differentiation can leave many cells unable to build a functional heart. The correct balance is spatial and temporal: different cardiac populations must be supplied, expand and mature in the right order.
Early cardiac mesoderm is specified through combinations of extracellular signals and transcription factors including GATA4, NKX2-5 and TBX5. The first heart field differentiates relatively early and contributes prominently to the initial heart tube and future left ventricle. The second heart field retains proliferative progenitor cells outside the tube for longer and adds cells at its poles, with major contributions to the right ventricle and outflow tract as well as other regions. These are useful developmental populations rather than perfectly isolated compartments with one exclusive marker. The key growth mechanism is delayed recruitment: maintaining a progenitor cell reservoir allows the heart tube to lengthen after its first contractile cells have differentiated.[ref]
FGF signalling helps support progenitor cell expansion, while BMP signalling contributes to specification and the transition toward differentiation. Their effects depend on developmental stage and location, so a global instruction to activate either pathway is inadequate. In mouse, an NKX2-5-dependent negative-feedback circuit limits Bmp2/Smad1 activity in heart-field progenitor cells. Nkx2-5 mutants initially overexpressed specification and progenitor cell programmes but subsequently failed to sustain normal second-heart-field proliferation and outflow-tract development. Reducing Smad1 activity rescued important aspects of these defects. The genetic rescue is stronger mechanistic evidence than an expression correlation: excessive specification-associated signalling can compromise the growth needed to construct the outflow tract.[ref]
Once incorporated into the heart, embryonic cardiomyocytes assemble sarcomeres and contribute to contraction while retaining substantial proliferative capacity. cell proliferation in this differentiated population thickens chamber walls and helps produce the tissue needed for septation. Chamber myocardium and non-chamber regions follow different regulatory programmes, allowing rapid chamber expansion alongside specialized conduction and junctional territories. The goal is not simply maximum cardiomyocyte number: the arrangement, coupling and regional identity of those cells are necessary for a coordinated pump.
Signals between cardiac layers couple growth to architecture. endocardium-derived neuregulin 1 acts through myocardial ErbB receptors, including ErbB2 and ErbB4, in ventricular trabeculation. Mouse loss-of-function experiments disrupting this ligand-receptor system produce severe defects in trabecular development. The phenotype demonstrates an essential tissue interaction, but absent trabeculae must not automatically be described as a pure proliferation defect: differentiation, adhesion, cell rearrangement and survival can also contribute. Separate measurements of these processes are needed.[ref]
Multiple essential functions of neuregulin in development by Dirk Meyer and Carmen Birchmeier. Targeted neuregulin mutation and embryonic cardiac phenotype
The epicardium and developing coronary system add further supporting signals and structural requirements as the ventricular wall grows. Proliferation must remain matched to oxygen delivery and tissue organization.Hippo signalling provides a direct brake on myocardial expansion. When active, the pathway restricts nuclear growth-promoting activity of YAP and its cooperation with TEAD factors. Conditional disruption of Hippo components in developing mouse hearts increased cardiomyocyte proliferation and enlarged the heart. Reducing beta-catenin dosage suppressed overgrowth in the tested mutants, supporting functional interaction with Wnt signalling. This demonstrates that differentiated myocardium contains an actively regulated growth programme; its number of divisions is not merely the residue of an earlier progenitor cell state.[ref]
Hippo pathway inhibits Wnt signaling to restrain cardiomyocyte proliferation and heart size by Todd Heallen and others. Cardiac conditional mutants, proliferation measurements and beta-catenin genetic interaction
Conversely, unrestricted proliferation is not necessarily desirable, because chamber geometry, septation and function must mature together.Around birth, cardiomyocytes undergo substantial changes in metabolism, sarcomere organization, electrical coupling and loading. Many mouse cardiomyocytes become binucleate or acquire polyploidy, while growth shifts increasingly toward cardiomyocyte hypertrophy. This transition is gradual and species-dependent, not a universal instantaneous switch at birth. A nucleus incorporating a nucleotide analogue may have undergone DNA replication without completing a new cell: endoreduplication and failed cytokinesis can mimic proliferation in a simple staining assay. Counts of total cardiomyocytes, nuclear number, DNA content and directly observed division are therefore needed alongside EdU and mitotic markers.
The early postnatal regeneration window illustrates the importance of developmental timing. Partial apex resection in one-day-old mice was followed by substantial myocardial restoration, and fate mapping implicated pre-existing cardiomyocytes; the reported capacity was greatly reduced by seven days of age. This is evidence that early differentiated cardiomyocytes retain regenerative potential under the tested injury conditions, rather than evidence for an indefinitely active adult cardiac stem-cell reservoir.[ref]
Transient regenerative potential of the neonatal mouse heart by Enzo R. Porrello and others. Age comparison, injury experiments and cardiomyocyte fate mapping
Injury severity and the method of measuring tissue restoration matter when comparing regenerative outcomes.To distinguish mechanisms experimentally, combine inducible lineage tracing with stage- and lineage-specific perturbation. Deleting a regulator before heart-field specification tests a different question from deleting it after cardiomyocyte differentiation. Follow progenitor cell number, recruitment, differentiated-cell number, completed division, apoptosis and chamber structure, then test pump function. Use littermate controls, verify recombination timing and specificity, and seek pathway-specific genetic rescue. A small heart with few marker-positive cells could reflect failed specification, reduced proliferation, delayed deployment or excess death. The developmental solution is an ordered handover: expand competent progenitor cells, recruit them into differentiated tissue, permit controlled division of working myocardium, and progressively constrain division as mature structure and function are established.
Polarity proteins generate tissue form by controlling where cells build surfaces, place junctions and divide. Their morphogenetic roles can be separated experimentally from a wholesale loss of epithelial identity. Three examples illustrate different outputs: positioning a single lumen, orienting neighbour exchange, and limiting tube dimensions.
The first example is Cdc42-dependent lumen formation in three-dimensional Caco-2 epithelial cysts. Cells in a normal cyst coordinate their apical-basal polarity so that apical surfaces face one central lumen. During growth, a correctly oriented spindle apparatus places daughter cells into the epithelial wall rather than establishing inappropriate internal cell arrangements. Cdc42 depletion disrupts spindle orientation and produces abnormal, often multiple, luminal spaces. Importantly, the cells can still establish apical membrane identity: in this model the crucial defect is the coordination and positioning of apical surfaces during division, rather than an absolute inability to make any apical surface. This distinguishes tissue-level organization from polarity within an isolated cell.[ref]
Cdc42 controls spindle orientation to position the apical surface during epithelial morphogenesis by Aron B. Jaffe and others. Caco-2 three-dimensional cysts, Cdc42 depletion and spindle-orientation analysis
Mechanistically, Cdc42 connects cortical organization to the PAR polarity complex, polarized trafficking and spindle-positioning machinery. However, the relative contributions depend on the model: a Cdc42 trafficking phenotype in another epithelial line cannot simply be substituted for the Caco-2 spindle result. A convincing test combines live-cell imaging of division and the first ectopic lumen with apical and basal markers, verifies target depletion and rescues with functional Cdc42. Compare the total number and viability of cells, because a dying cell population can also produce abnormal cavities. A perturbation that restores spindle positioning while leaving other outputs of Cdc42 impaired would help isolate the causal route. These controls make the single-lumen phenotype an interpretable morphogenetic output.
The second example is Bazooka, the fly PAR-3 protein, during Drosophila germband extension. This uses planar cell polarity within the epithelial sheet as well as apical-basal organization. Bazooka and junctional components become enriched at a complementary set of cell interfaces to myosin II. Spatially patterned gene activity organizes this planar asymmetry, and loss of Bazooka disrupts normal polarized cell behaviour and extension. Thus a protein associated with epithelial junction assembly is redeployed to make different junctions behave differently in the same sheet.[ref]
Patterned gene expression directs bipolar planar polarity in Drosophila by Jennifer A. Zallen and Eric Wieschaus. Planar distributions of Bazooka and myosin and dependence on patterned gene expression
Oriented junction shrinkage and new-junction formation permit cell intercalation while maintaining epithelial continuity. The important geometry is that junctions separating anterior and posterior neighbours shrink and resolve into interfaces with the complementary orientation, producing extension along the body axis. Junction names can be confusing because they may describe either the neighbours or the line itself; tracking vertices and neighbour exchange avoids this ambiguity. Bazooka is a spatial organizer, not itself the force-generating motor. To test its contribution, quantify its localization, myosin localization, junction lifetimes, cell rearrangements and tissue strain after an acute or mosaic perturbation that leaves enough epithelial structure for movement to occur. A general epithelial collapse would establish an essential structural role but would not isolate its role in planar coordination.
The third example is control of fly tracheal tube size by the apical determinant Crumbs and basolateral regulators including Yurt and Coracle. Crumbs promotes the apical domain, so restricting its activity helps constrain the amount of luminal cell surface and hence tube dimensions. Mutations in yurt produce overlong tracheal tubes, and reducing Crumbs dosage suppresses important length defects; Crumbs overexpression has the opposite tendency. This genetic interaction connects the balance of apical and basolateral regulators to organ geometry rather than simply to the presence of an epithelial sheet.[ref]
Epithelial polarity proteins regulate Drosophila tracheal tube size in parallel to the luminal matrix pathway by Patrick Laprise and others. Tube measurements, Crumbs dosage suppression and Vermiform secretion controls
The luminal extracellular matrix is a crucial control in this example. Septate-junction-associated proteins can also affect delivery of the matrix-modifying protein Vermiform, potentially changing tube shape indirectly. Yet yurt mutants retain Vermiform secretion, and reducing Crumbs can suppress coracle length defects without restoring the secretion defect. Scribble mutants also show long tubes but are not equivalently rescued by the tested Crumbs reduction. The result supports parallel and partly distinct routes, rather than a universal linear pathway in which every basolateral protein merely inhibits Crumbs. Compare cell number, apical area, tube length and diameter independently: a longer tube need not result from extra divisions. Quantitative dosage interactions and rescue are particularly informative because they can reveal a size-control function while preserving much of epithelial organization.
Together, these examples link polarity to three separable operations. Cdc42 coordinates the location of new apical surfaces during division; Bazooka contributes to directional junction remodelling within a sheet; and the Crumbs-regulator balance sets the extent of a luminal surface. Conversely, changing forces and geometry can alter junctional organization, so the relationship is reciprocal. The common principle is that epithelial polarity supplies spatial constraints on growth and rearrangement. It is a dynamic component of morphogenesis, not merely a static property to be established before morphogenesis starts.
Mechanics shapes tissues by generating active forces, directing rearrangements and converting constrained growth into deformation. Three experimentally distinct examples are folding of the fly ventral epithelium, elongation of the fly germband and formation of chick intestinal villi. They respectively emphasize changes in cell shape, changes in cell neighbours and a growth-driven instability. In each case, a satisfactory explanation needs both a force-generating process and the material or boundary conditions that convert it into a particular shape.
First, apical constriction drives Drosophila ventral furrow formation. Ventral cells accumulate a contractile actomyosin network near their apical surfaces. Reducing apical area while retaining tissue continuity changes cell geometry and contributes to inward bending of the epithelial sheet. This is not adequately described as uniform contraction of a permanent circumferential belt. Time-resolved imaging showed pulses of medioapical myosin II accumulation associated with discrete contractions, and stabilization between pulses permits net constriction. Regulation by Snail and Twist helps coordinate contraction and the retention of the resulting shape.[ref]
Pulsed contractions of an actin-myosin network drive apical constriction by Adam C. Martin and others. Live imaging, pulsatile apical contraction and transcription-factor perturbations
The force must be transmitted to neighbouring cells through adherens junctions; a detached contracting cortex can deform internally without folding a coherent sheet. Geometry is therefore a collective property. A useful causal test compares acute inhibition of myosin activation with perturbation of junctional coupling, scoring apical area, contraction pulses, cell length and tissue curvature separately. laser ablation can reveal the direction of tissue load, and localized activation of contractility can test whether the site of force generation predicts bending. Recoil velocity alone is not tension: in an overdamped approximation , where is released tension and an effective resistance. Comparing recoil between conditions requires considering possible changes in resistance as well as load. External pressure, basal constraints and neighbouring tissue movement also influence invagination, so apical contraction need not be sufficient under every boundary condition.
Second, Drosophila germband extension changes tissue aspect ratio through oriented cell intercalation. Selected cell junctions shrink, cells briefly share a vertex or multicellular rosette, and new junctions appear in the complementary orientation. Repeated local neighbour exchanges extend the tissue along one axis while narrowing it along the other. myosin II is enriched at the shrinking interfaces, and interfering with its activity disrupts polarized junction remodelling. This supplies a mechanism for convergent extension without requiring that every cell grow longer or that an increased number of divisions provide the extension.[ref]
Myosin-dependent junction remodelling controls planar cell intercalation and axis elongation by Claire Bertet and others. Time-lapse junction analysis and perturbation of polarized myosin activity
Here the crucial distinction is between active rearrangement and passive stretching. Track all vertices and neighbours in a patch and decompose tissue deformation into cell-shape change, neighbour exchange and cell-number change. A tissue can lengthen while individual cells remain similar in shape if topology changes; alternatively, pulling from a neighbouring tissue can elongate cells without local intercalation supplying the force. Test whether local myosin inhibition suppresses the junction transitions before global tissue movement is lost, and compare spatial patterns of load by laser ablation. Rescue must restore directional transitions as well as the final length. planar cell polarity provides the orientation, and junctional adhesion permits force transmission while contacts are remodelled. Thus mechanics can translate a molecular anisotropy into coordinated movement of an epithelial sheet.
Third, chick intestinal villi illustrate differential growth constrained by surrounding layers. The growing inner tissues are enclosed by sequentially differentiating smooth muscle layers. Mechanical constraints drive a progression from longitudinal ridges through zigzags toward a villous surface. The important process is not simply muscle contraction pushing each villus into place: the muscle acts as a restricting layer against which continued tissue growth builds compressive stress. In the primary experiments, blocking muscle differentiation prevented the expected folding, while an artificial constraining silk tube could restore folding in the inhibited tissue. This rescue is particularly informative because it replaces a living layer's mechanical contribution without restoring all its possible signals.[ref]
Villification: how the gut gets its villi by Amy E. Shyer and others. Muscle perturbation, artificial confinement and mechanical modelling
The physical principle is a buckling instability: a sufficiently compressed growing layer can lower its mechanical cost by bending. The wavelength and mode depend on geometry, thickness and stiffness, so equal amounts of growth need not yield equal shapes in different environments. An ideal thin-plate model has bending rigidity , with Young's modulus , thickness and Poisson's ratio . It predicts strong thickness sensitivity of resistance to bending, but this formula alone does not compute the wavelength of a living multilayer gut. That requires measured geometry, growth and an appropriate constitutive model. Compare proliferation, muscle differentiation, material properties and folding after each perturbation to distinguish mechanical confinement from secondary effects on growth.
The chick example should not be imposed unmodified on mouse villus development, where mesenchymal cluster patterning precedes the corresponding epithelial deformation. Nor is any of the three mechanisms independent of chemical signalling: signals position contractility, specify muscle and regulate adhesion, while mechanical deformation changes the subsequent signalling environment. Their distinct causal signatures are nonetheless clear. A contractile apical network folds a coupled sheet; anisotropic junctional tension changes neighbours and tissue aspect ratio; constrained growth generates an instability whose form depends on material properties. Testing these signatures through timed perturbation and mechanical rescue explains organ shape more precisely than simply observing that a cytoskeletal protein is required.
taphonomic bias is systematic distortion of biological information between a living community and the fossil record. Death, carcass decay, scavenging, transport, burial, chemical alteration, exposure and collection all filter what is observed. A deposit therefore samples organisms, body parts and environments unequally. This is more than incompleteness: preferential preservation of a particular tissue or habitat can produce a misleading pattern of abundance, anatomy or evolutionary timing.
An autochthonous fossil assemblage contains remains preserved where the organisms lived; an allochthonous fossil assemblage contains material transported from elsewhere. These describe provenance, rather than two levels of fidelity. In an allochthonous fossil assemblage, currents can separate elements by size, shape and density, concentrate resistant teeth or scales, remove delicate bodies and mix organisms from different habitats. Erosion and redeposition can also introduce older fossils into younger sediment. Such reworking differs from simple transport of recently dead animals. time averaging mixes deaths from different times even without long-distance transport. A concentration of robust remains consequently need not represent either a locally abundant living population or a single ecological event.
An autochthonous fossil assemblage avoids some transport distortion, but still selects organisms and characters. A bottom-dwelling community rapidly buried in place can be unusually well represented while swimmers above it, unmineralized tissues and organisms living outside that depositional setting are missing. Conversely, an intact carcass can travel before burial, whereas locally decayed remains can become disarticulated without transport. Articulation, abrasion, preferred orientation, sedimentary context and age agreement must therefore be evaluated together. Local preservation does not imply an unbiased biological census.
The contrast between cyclostomes and early members of the gnathostome lineage is particularly revealing. Living cyclostomes, hagfish and lampreys, have no extensive mineralized external skeleton comparable to the armour of many early jawless relatives of gnathostomes. Their bodies are dominated by tissues whose preservation usually requires exceptional conditions. The abundance of isolated mineralized scales, plates or teeth can thus make a hard-bodied lineage conspicuous where a soft-bodied contemporary is virtually invisible. Importantly, the armoured jawless assemblage traditionally called ostracoderms is not simply the ancestral cyclostome record: many of its members belong on the gnathostome stem. Absence of jaws does not by itself establish cyclostome affinity.
There is also a character-level filter. Robert S. Sansom and colleagues followed experimental carcass decay of living chordates, and then examined hagfish and lampreys in detail. Anatomical characters did not disappear at random: loss of diagnostic features could make a derived animal appear more primitive. This produces stemward slippage if investigators mistake an unpreserved feature for a feature absent in life. The result is relevant both to isolated soft-bodied fossils and to the apparently long primitive intervals preceding well-preserved groups.[ref]
Non-random decay of chordate characters causes bias in fossil interpretation by Robert S. Sansom and others. Experimental character-loss sequences and simulated consequences for fossil interpretation
[ref]Decay of vertebrate characters in hagfish and lamprey (Cyclostomata) and the implications for the vertebrate fossil record by Robert S. Sansom and others. Comparative decay of cyclostome tissues and diagnostic characters
A useful experimental design records fresh anatomy first, samples replicated carcasses through time under stated temperature and chemical conditions, and scores the same characters in each specimen. Comparisons between animals and between preservational conditions test whether the loss order is reproducible. Such experiments identify plausible biases; they do not recreate every burial chemistry or prove that every uncertain fossil has undergone the same sequence. In a phylogenetic character matrix, genuinely unobservable anatomy should normally be coded as unknown rather than automatically absent. Comparison across differently preserved specimens can sometimes recover information that one specimen lacks.
Exceptional discoveries show what the ordinary record omits. The Late Devonian lamprey Priscomyzon from South Africa preserves a recognizable oral apparatus and branchial region without a massive mineralized skeleton. It shows that early lamprey anatomy can be recovered when the appropriate soft-tissue window is available; the gap before such a discovery is not evidence that the lineage had just originated.[ref]
A lamprey from the Devonian period of South Africa by Robert W. Gess and others. Description and Late Devonian occurrence of Priscomyzon
The Cretaceous hagfish Tethymyxine preserves evidence including slime-producing structures, allowing characters unavailable in most older deposits to be brought into an analysis using phylogenetics. It supplies a minimum occurrence and anatomical information, not the date when hagfish originated.[ref]Hagfish from the Cretaceous Tethys Sea and a reconciliation of the morphological–molecular conflict in early vertebrate phylogeny by Tetsuto Miyashita and others. Fossil anatomy, slime-gland evidence and combined phylogenetic analysis
Conversely, Early Silurian Qianodus is known through mineralized tooth whorls: such durable small remains can establish an early occurrence of a toothed gnathostome even where complete bodies are missing.[ref]The defensible comparison concerns preservation probabilities as well as biological histories. First fossil occurrences are minimum ages, and unequal counts need not measure unequal diversity. Independent anatomical characters, comparable depositional settings, searches for small hard parts and exceptional soft-tissue deposits together give a better test of early vertebrate history than a literal reading of the most conspicuous remains.
The transition places vertebrate origins within a prolonged assembly of animal body plans, ecological interactions and preservational opportunities. It does not identify one boundary at which a complete modern vertebrate suddenly appeared. Three questions must be separated: when the relevant lineages diverged, when diagnostic features evolved, and when those features became recoverable as fossils.
The Ediacaran precedes the Cambrian, whose beginning is approximately 539 million years ago. Ediacaran communities already contained macroscopic organisms and evidence of animal movement and feeding. Kimberella, for example, has been interpreted from its body organization as a mollusc-like bilaterian; its relevance is that substantial animal differentiation predates the boundary, rather than that it is a vertebrate ancestor.[ref]
The Late Precambrian fossil Kimberella is a mollusc-like bilaterian organism by Mikhail A. Fedonkin and Benjamin M. Waggoner. Body reconstruction and bilaterian interpretation
trace fossils record activities that may otherwise leave no body remains. Increasingly elaborate movement and sediment disturbance reveal ecological capacities, but an isolated burrow does not identify a notochord, a head or a particular branch of the animal phylogenetic tree.Across the transition, animal skeletons, predation, burrowing and water-column communities became more prominent. Their appearance changes both biology and observation. Resistant skeletons improve preservation, while bioturbation can destroy the sedimentary surfaces that had preserved some earlier soft-bodied communities. Different preservational windows reveal different subsets of life. An apparent replacement in the fossil record can therefore combine real ecological turnover with taphonomic bias. One should compare anatomy and environments across several deposits rather than treating all Ediacaran absences as biological absences.
The Cambrian exceptional deposits provide positive evidence. Haikouichthys and Myllokunmingia from Chengjiang reveal small fish-like animals with combinations of axial, muscular and branchial structures interpreted as early vertebrate organization.[ref]
Lower Cambrian vertebrates from south China by D.-G. Shu and others. Descriptions and reconstruction of the two Chengjiang taxa
Metaspriggina from the Burgess Shale adds evidence from a distinct assemblage, including prominent eyes, segmented musculature, organized into myomeres, and serial branchial supports.[ref]A primitive fish from the Cambrian of North America by Simon Conway Morris and Jean-Bernard Caron. Anatomical description and reconstruction of Metaspriggina
These are more informative than an undifferentiated claim that “fish existed”: they allow particular characters to be mapped onto alternative phylogenetic trees.A plausible sequence involves a swimming chordate organization with a notochord and segmental musculature, followed by elaboration of anterior sensory and feeding systems along the vertebrate lineage. Nevertheless, fossil compressions can obscure boundaries or superimpose unrelated structures. Confidence should come from repeated specimens, bilateral agreement, positional relationships and combinations of characters, rather than resemblance of one dark patch to an organ. A structure absent from a compressed specimen may be unpreserved. Nor does a plausible early vertebrate have to be a member of the living vertebrate crown group, still less a direct ancestor of a living species. A stem group can contain extinct side branches showing different combinations of ancestral and derived states.
Living organisms constrain the reconstruction without forming a ladder. Molecular analyses place tunicates, rather than cephalochordates, as the closest living relatives of vertebrates.[ref]
Tunicates and not cephalochordates are the closest living relatives of vertebrates by Frédéric Delsuc and others. Phylogenomic comparison of chordate relationships
A modern lancelet is consequently a comparative relative with its own history, not an unchanged stage through which vertebrates passed. The same warning applies to living hagfish and lampreys. Their anatomy can reveal inherited features and secondary specializations; simplicity alone cannot polarize a character.The New Head hypothesis connects cranial sensory and feeding innovations with neural crest and ectodermal placodes. This is a developmental explanation for assembling a more elaborate head. Experiments on living chordates can test where cells originate, which structures they form and which regulatory interactions are needed. The fossil presence of eyes or branchial supports cannot directly demonstrate the embryonic migration of neural crest. Conversely, a conserved regulatory gene alone does not establish that a complete modern head existed in an Ediacaran ancestor. Developmental, molecular and anatomical evidence address complementary parts of the argument.[ref]
Neural crest and the origin of vertebrates: a new head by Carl Gans and R. Glenn Northcutt. Proposed developmental basis and functional significance of head innovation
Ecological context helps explain why these capacities might diversify. More active swimming, prey detection and food processing can create opportunities and selective pressures for improved sensory and locomotor coordination. molecular oxygen availability constrains the metabolic activities that can be sustained. Erik A. Sperling and colleagues compared modern low-oxygen animal communities and related the scarcity of carnivory at low oxygen levels to hypotheses about Cambrian ecological expansion.[ref]
Oxygen, ecology, and the Cambrian radiation of animals by Erik A. Sperling and others. Modern oxygen-gradient observations and the proposed ecological connection
This motivates a mechanism; environmental correlation alone neither dates the vertebrate ancestor nor establishes oxygenation as a sufficient single cause.The useful conclusion is a constrained historical sequence, with explicit gaps. Ediacaran evidence establishes antecedent animal complexity; Cambrian exceptional preservation documents recognizable early vertebrate combinations; comparative phylogenetics and evolutionary developmental biology test their placement and assembly. molecular clocks can estimate earlier divergences, but their dependence on rates and fossil calibration prevents them from turning every absence into a precise origin date.
Sarcopterygii is the clade comprising the most recent common ancestor of living coelacanths, lungfish and tetrapods, together with all its descendants. In this crown-based usage, humans are sarcopterygians: acquisition of limbs and loss of a fish-like outline do not remove descendants from a clade. Extinct taxa assigned along the stem require an explicitly broader total-group usage. A diagnosis lists characters useful for recognizing a group; a synapomorphy is a shared derived character whose position has been inferred on a phylogenetic tree. Those are related but not interchangeable statements.
Two particularly instructive traditional diagnostic features are the fleshy, internally supported paired appendages and true enamel associated with the dentition. The first survives conspicuously in our arms and legs. The second survives in our tooth crowns, although modern evidence requires qualification of its traditional status as an exclusively sarcopterygian innovation.
The paired-appendage transformation. A lobed fin contains musculature and a substantial endoskeleton extending into the appendage. In the relevant ancestral pattern, a single proximal skeletal element connects to the girdle: the humerus in the pectoral appendage, and the femur in the pelvic appendage. Subsequent elements elaborate the jointed internal axis. The important comparison is historical organization and articulations, not merely that both a fin and an arm contain bone. fins in other lineages also possess internal supporting elements, so the presence of any fin skeleton is too broad a diagnosis.
Within the lineage leading to tetrapods, the pectoral series can be recognized as humerus, radius bone and ulna, followed by increasingly elaborate distal elements. Tiktaalik retains fin rays but has a distal jointed skeleton capable of limb-like positioning against a substrate. Its combination of characters shows that parts of a wrist-like support system preceded a fully digit-bearing hand. Comparing several articulated specimens and the geometry of joint surfaces constrains the reconstruction better than matching isolated bones by outline.[ref]
The pectoral fin of Tiktaalik roseae and the origin of the tetrapod limb by Neil H. Shubin and others. Pectoral anatomy, joint configurations and proposed substrate-supported postures
Further changes included anatomical digits, loss of external fin rays in the limb, changes to the girdles and altered force transmission through the trunk. They did not all arise simultaneously. Early digit-bearing tetrapods were not uniformly five-fingered terrestrial walkers; aquatic settings and polydactyly make it misleading to present the modern human hand as the immediate purpose or original endpoint of the transition. Acanthostega, with eight anatomical digits in its forelimb, supplies a concrete counterexample to an ancestrally universal five-digit condition.[ref]
Polydactyly in the earliest known tetrapod limbs by Michael I. Coates and Jennifer A. Clack. Digit counts and implications for the ancestral tetrapod limb
Our own upper limb retains the proximal single-bone and paired-bone organization, but the shoulder, elbow, wrist and fingers are extensively specialized. Rotation of the radius bone relative to the ulna contributes to turning the forearm; an opposable thumb and independently controlled fingers support grasping. In the lower limb, the femur, tibia and fibula show the corresponding serial organization, while the pelvis, hip, knee and foot transmit loads in habitual bipedalism. These are derived modifications within tetrapods, rather than defining traits of all Sarcopterygii. Comparing our arm with a fish pectoral fin concerns biological homology between organisms; comparing arm and leg also involves serial homology within the body.
The dental transformation and its qualification. human tooth crowns have an outer layer of enamel over dentine. enamel is highly mineralized and is produced by epithelial ameloblasts, whereas dentine is a different tissue formed by odontoblasts. Identifying a fossil surface as enamel therefore requires tissue architecture and developmental or molecular comparison, not simply a shiny hard covering. In our teeth the coating has specialized organization into enamel rods and contributes to wear resistance during biting and chewing. tooth classes and crown shapes diversify the ancestral feeding apparatus; they are not themselves basal sarcopterygian synapomorphies. After eruption, loss of the enamel-producing cellular layer severely limits biological replacement of worn crown enamel.
The traditional contrast between sarcopterygian true tooth enamel and other hard coverings needs an explicit historical correction. Qingming Qu and colleagues combined fossil histology with evidence for enamel-matrix genes in the skin of gar. In Psarolepis, external odontodes carried enamel while the teeth lacked an enamel coating. Their evidence supported an origin in dermal coverings followed by expansion into the mouth, and an ancestry deeper than Sarcopterygii alone.[ref]
New genomic and fossil data illuminate the origin of enamel by Qingming Qu and others. Fossil tissue distribution and gar enamel-matrix gene expression
Thus enamel and its oral deployment must be coded separately; tooth enamel remains a useful traditional diagnostic comparison, but the tissue itself is not a uniquely sarcopterygian synapomorphy. Shared tissue can undergo heterotopy, loss and later modification.The two histories illustrate different forms of transformation visible in our bodies: an internally supported paired fin became a jointed, digit-bearing, specialized limb, and an inherited mineralized epithelial covering acquired a complex role in our dentition. A rigorous diagnosis states the anatomical level being compared and distinguishes inherited organization from later functional specialization. Neither the modern function nor the external human appearance determines membership of Sarcopterygii.
A monophyletic group includes an ancestor and all its descendants; a paraphyletic group includes an ancestor but excludes some descendants; a polyphyletic group combines separate lineages while excluding their relevant common ancestry. The distinction concerns how membership relates to a phylogenetic tree, rather than how many visible similarities the members possess.
Consider a simplified tree of living amniotes: mammals form one branch, while the other contains lepidosaurs, turtles and archosaurs; living archosaurs comprise crocodilians and birds. Within the latter branch, birds are surviving dinosaurs. The tree below omits extinct branches and most living diversity, and its branch lengths represent neither age nor quantity of evolutionary change. It illustrates three choices of group on the same ancestry.
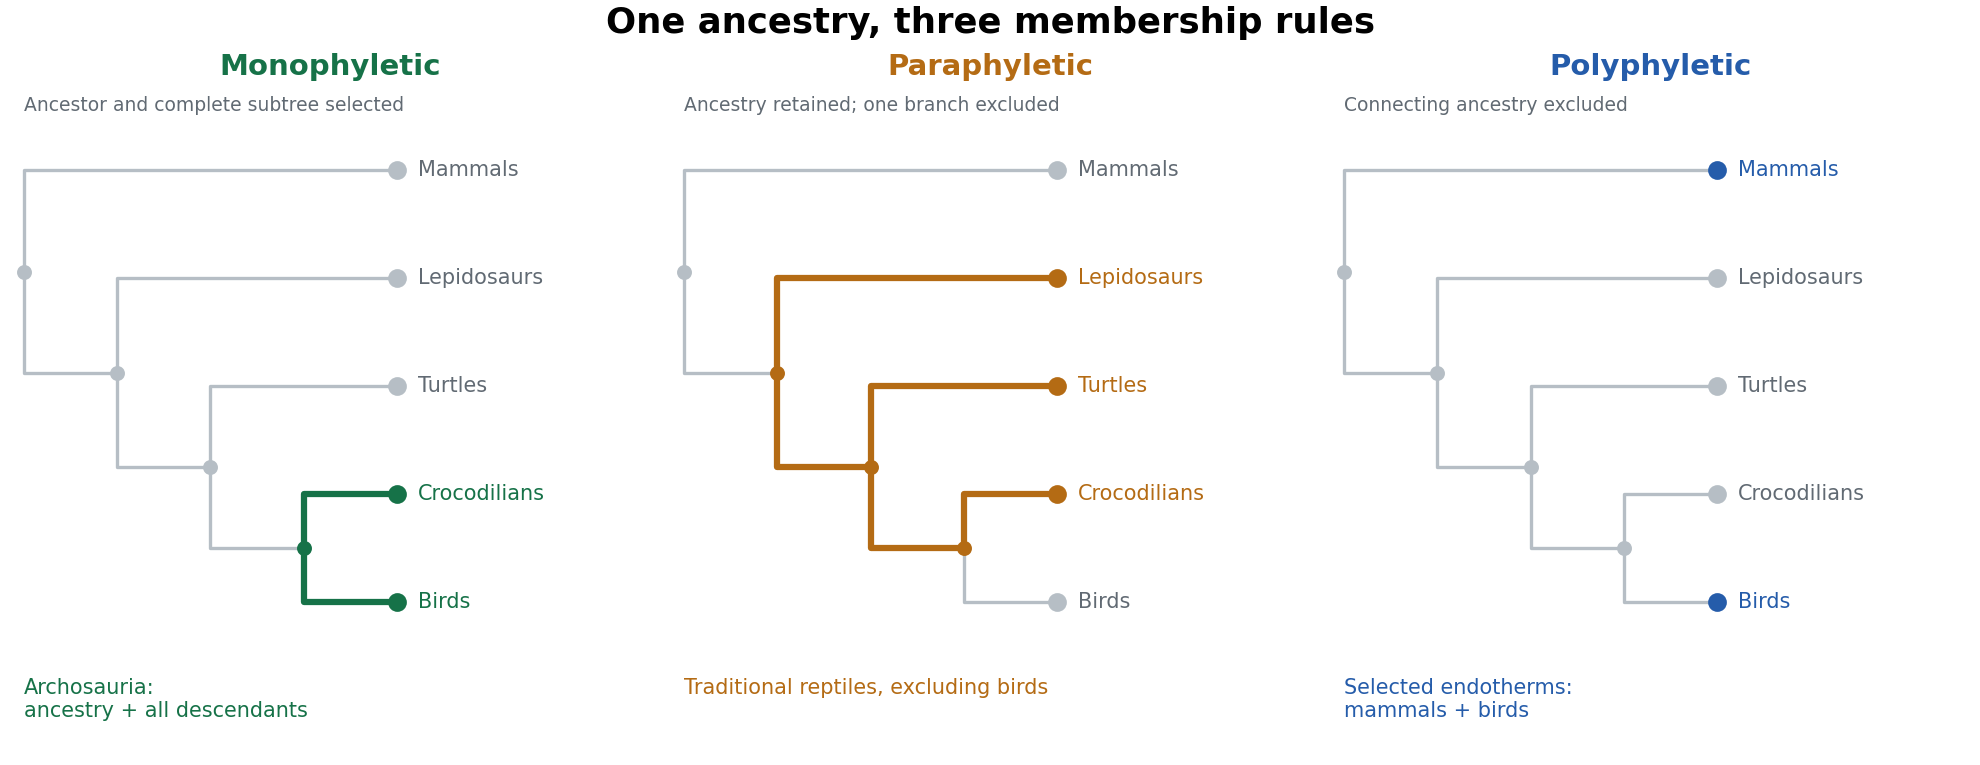

A monophyletic group is a clade. Archosauria includes the last common ancestor of birds and crocodilians and every descendant, including extinct dinosaurs and other extinct branches. In the simplified figure, selecting their shared node and both descendant tips gives the corresponding complete subtree. Sarcopterygii, with tetrapods included, is another example. A clade need not be recognized by a feature that remains visibly unchanged in every descendant: subsequent modification and loss are permitted. It also need not have a particular taxonomic rank.
A familiar paraphyletic group is the traditional assemblage “reptiles” when it includes turtles, lizards, snakes and crocodilians but explicitly excludes birds. The latter descend from within the ancestry otherwise assigned to that assemblage. The selected ancestry is therefore cut short at one of its own branches. Similarly, conventional “fish” that include finned sarcopterygians but exclude tetrapods form an evolutionary grade rather than a complete clade. These examples require the stated usage: Reptilia or Sauropsida can instead be defined as a clade that includes birds. The everyday word does not irrevocably determine the phylogenetic status of every technical definition bearing that name.
For polyphyly, consider assembling mammals and birds solely as the familiar independently evolved examples of sustained high metabolic heat production, while omitting their intervening ancestors and other descendants. This physiological grouping can be useful for comparing endothermy, but it does not identify one exclusive historical lineage. Their last common ancestor also has descendants such as lepidosaurs and crocodilians. On the usual inference of independent elaboration of the relevant physiology, the selected resemblance involves convergent evolution. Calling the assemblage “warm-blooded vertebrates” must not turn a selected physiological trait into evidence that birds are closer to mammals than to crocodilians. Moreover, endothermy and constant body temperature are not identical properties, and living taxon sampling does not locate every thermophysiological transition in extinct lineages.
There is a subtle distinction between the last two cases. A diagram of selected terminal tips alone can show that a group is not a clade, but does not always uniquely distinguish paraphyly from polyphyly. One must state which ancestors are included and the historical interpretation of the defining character. In the orange example, the ancestral reptile lineage is retained and one descendant branch excluded. In the blue example, similar functional outcomes are assembled from separate branches without including the connecting ancestry. The highlighted internal paths in the figure make that difference explicit.
clades are particularly suitable for discussing vertebrate evolution because their nested membership directly expresses common descent. They permit consistent statements such as “birds are dinosaurs” and “humans are sarcopterygians”, while allowing substantial changes in form and function. Shared derived characters, or synapomorphies, provide evidence for branches; shared ancestral states do not uniquely diagnose the smaller groups inheriting them, and independently acquired similarities require separate explanation. This framework makes character transformations testable against a branching history instead of arranging animals in a ladder of increasing complexity.
In practice the phylogenetic tree remains a hypothesis. More characters, better fossils or different evolutionary models can change inferred relationships. Naming a clade with an explicit ancestry-based definition helps keep the statement intelligible when that happens, but does not make the inference immune to error. Anatomical and molecular characters need biological homology assessment, appropriate taxon sampling and uncertainty estimates. For example, genome-scale data and stem-turtle anatomy independently address whether turtles lie near archosaurs, rather than treating one skull condition as sufficient to define the tree.[ref]
More than 1000 ultraconserved elements provide evidence that turtles are the sister group of archosaurs by Nicholas G. Crawford and others. Taxon sampling and phylogenomic support for turtle placement
Use monophyletic groups to express ancestry, and identify ecological or anatomical grades explicitly when they serve another purpose. paraphyletic groups can summarize retained ancestral organization, and polyphyletic groups can support functional comparisons, but neither should silently substitute for a complete lineage.
The avian digit identity frameshift hypothesis proposes that positional condensations conventionally numbered II, III and IV develop morphological identities I, II and III. It separates the place where an anatomical digit develops from the inherited developmental identity expressed there. It is a hypothesis about evolutionary developmental biology, not a frameshift mutation in a DNA reading frame.
The problem arose from comparing two kinds of evidence. The hands of the theropod relatives of birds were traditionally reconstructed as retaining the first three anatomical digits. Their bone relationships and, in appropriate fossils, the phalangeal pattern of two, three and four phalanges supported identities I, II and III. Embryological studies of the bird wing instead assigned the principal surviving condensations to positions II, III and IV within a pentadactyl reference pattern, partly from their relation to the primary skeletal axis. If positional number necessarily fixed morphological identity, the interpretations appeared inconsistent.
biological homology is a historical claim, however, and a developmental coordinate need not be eternally coupled to the same character identity. Günter P. Wagner and Jacques A. Gauthier proposed an evolutionary change in that coupling: an anatomical digit formed at position II could execute an identity-I developmental program, and the two posterior anatomical digits could undergo the corresponding changes.[ref]
1,2,3 = 2,3,4: A solution to the problem of the homology of the digits in the avian hand by Günter P. Wagner and Jacques A. Gauthier. The developmental frameshift proposal reconciling positional and morphological assignments
With denoting a positional condensation and its resulting identity, the classical proposal is:This notation describes a change in specification. It does not mean that a fully formed thumb physically migrated into another anatomical digit's position during development.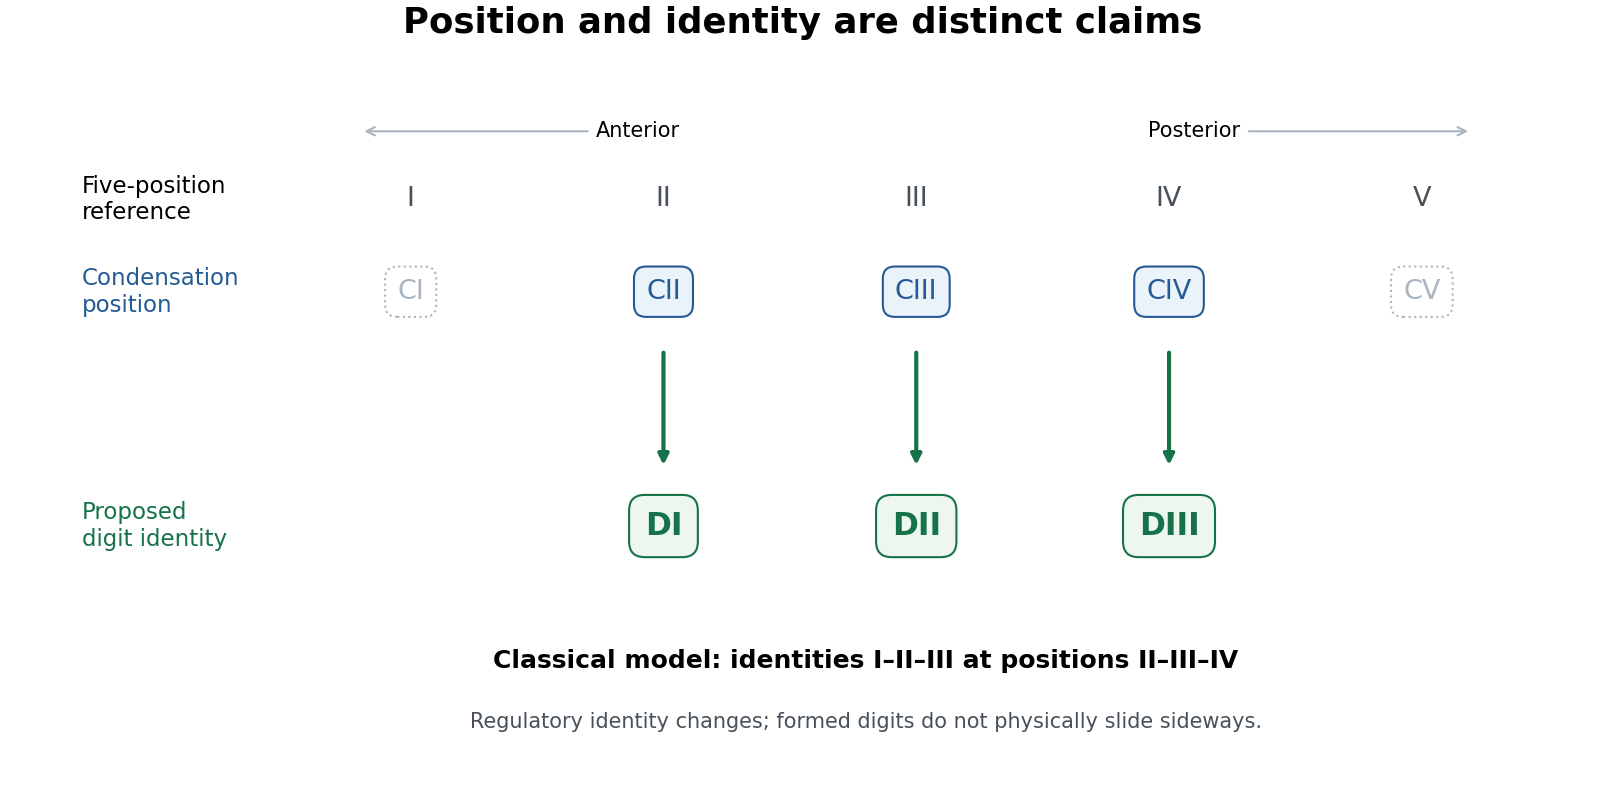
Positional condensations and morphological identities in the classical avian digit frameshift hypothesis
. Original conceptual diagram. The upper row is a five-position reference; the lower rows distinguish the retained positional assignments from the identities proposed for them. Dotted symbols indicate positions outside the three principal retained digits, without asserting that no transient cells or condensations ever occur there. This diagram states the classical model, not a universal molecular identity code. Details.
The proposal yields tests. Anatomical identity should be assessed from several features of metacarpals, joints and phalanges, not by calling the anteriormost remaining anatomical digit “I” by definition. Condensation position should be established independently from staged embryos and fate mapping, rather than inferred solely from the adult hand. Molecular comparisons can then ask whether positional anatomical digit II in the wing shares a distinctive regulatory state with anatomical digit I in a reference limb. evolution of gene regulation, including the duration and distribution of Sonic hedgehog signalling and downstream interactions, offers a means of uncoupling position and later differentiation. Expression of one Hox gene is informative but is not a universally valid barcode of a complete digit identity.
Koji Tamura and colleagues used cell labelling and transplantation to compare wing and hindlimb development. The cells contributing to the posterior wing anatomical digit did not have the same relationship to the posterior signalling region, the zone of polarizing activity, as the corresponding hindlimb anatomical digit IV; their early separation was compatible with a digit-III developmental domain. This supplied experimental evidence against equating the posterior wing anatomical digit straightforwardly with hindlimb anatomical digit IV.[ref]
Embryological evidence identifies wing digits in birds as digits 1, 2, and 3 by Koji Tamura and others. Cell-labelling and transplantation comparisons of wing and hindlimb digit progenitors
Such experiments need embryos matched by developmental stage, verified label positions, assessment of label persistence and spread, and controls for effects of grafting on survival and growth. A cell's ultimate contribution establishes its fate under the tested conditions; it does not alone establish the evolutionary identity of every structure it forms. Comparing forelimb with hindlimb also requires recognizing that the two are already developmentally different organs. The stronger inference combines lineage tracing with anatomy and regulatory evidence.
Transcriptomic data sharpened, rather than simply ended, the debate. Zhe Wang and colleagues found a conserved anterior-digit signature consistent with identity I in the anteriormost wing anatomical digit, while the posterior wing anatomical digits showed derived expression identities rather than a simple conserved series.[ref]
Transcriptomic analysis of avian digits reveals conserved and derived digit identities in birds by Zhe Wang and others. Comparative digit transcriptomes and the distinctive anterior-wing-digit signature
A later multi-species comparison by Thomas A. Stewart and colleagues challenged the assumption that all corresponding anatomical digits possess a conserved tetrapod-wide molecular identity. Their results supported a more limited shift rather than treating every posterior anatomical digit as an unchanged identity displaced by one position.[ref]Evidence against tetrapod-wide digit identities and for a limited frame shift in bird wings by Thomas A. Stewart and others. Cross-species expression comparisons and limits of a universal digit-identity model
Tissue composition, sampling stage, orthology assignment and the choice of reference species are therefore essential controls in molecular tests.The evolutionary significance is substantial but bounded. birds are nested within theropod dinosaurs on evidence extending beyond anatomical digit number, including many skeletal transformations and feathered relatives. The preserved integument of Yutyrannus, for example, documents filamentous feathers in a nonavian tyrannosauroid, broadening the fossil distribution of feathers beyond birds.[ref]
A gigantic feathered dinosaur from the Lower Cretaceous of China by Xing Xu and others. Associated skeletons and filamentous feather preservation in Yutyrannus
A coherent developmental mechanism removes one apparent contradiction between embryology and that historical interpretation. It also illustrates why disagreement between positional and morphological evidence should trigger a mechanistic test rather than automatic rejection of either dataset. However, showing that a regulatory shift is developmentally possible is not proof that precisely the full classical shift occurred in the ancestral bird lineage.The durable result is that anatomical digit position and digit identity can evolve partly independently. Evidence for an identity-I anterior wing anatomical digit is stronger than a claim that all three anatomical digits retain invariant molecular identities I, II and III. The digit identity frameshift hypothesis remains a useful, testable bridge between fossil anatomy and development, with the exact extent and sequence of identity transformation requiring explicit comparison rather than assumed equivalence.
The turtle problem is the difficulty of placing turtles on the reptile phylogenetic tree, historically intensified by conflict between their unusual skulls and other anatomical or molecular evidence. Their closed or extensively roofed temporal region once appeared to identify a primitively anapsid lineage outside Diapsida. Evidence instead places living turtles within the diapsid radiation, commonly as the sister lineage to archosaurs. The inference requires distinguishing retention of an ancestral state from secondary modification.
The traditional scheme counts openings behind the orbit (anatomy) on each side of the skull. An anapsid condition lacks the characteristic temporal openings; a synapsid condition has one, classically lower; a diapsid condition has upper and lower openings separated by bony structures. These descriptions originally provided convenient anatomical categories. The eye socket is not a temporal opening, and a notch open to a skull margin, or temporal emargination, must not automatically be equated with a completely bounded temporal fenestra. bone identities and contacts matter as much as the count.
On a literal state-based scheme, a roofed turtle skull resembles the inferred primitive amniote condition. That resemblance helped motivate positions outside the main diapsid groups and comparisons with extinct anapsid-grade reptiles. Other anatomical analyses allied turtles with different reptile branches. Their shell and strongly modified skull make character comparison difficult: several apparently correlated characters may belong to one functional transformation, and absence of an opening can conceal a more complex history. A shared absence is especially weak evidence when the opening can be closed independently.
Molecular evidence provides an independent character system. Nicholas G. Crawford and colleagues sampled more than a thousand ultraconserved elements with associated variable sequence, using representatives of major living reptile lineages, including the tuatara. Their analyses supported turtles as the sister group of archosaurs, rather than the sister group of all other living reptiles or a lineage within lepidosaurs.[ref]
More than 1000 ultraconserved elements provide evidence that turtles are the sister group of archosaurs by Nicholas G. Crawford and others. Nuclear-locus sampling, inclusion of tuatara and inferred turtle–archosaur relationship
In this hypothesis, crocodilians and birds are closer to one another than either is to turtles. The schematic in solution 4 shows that distinction: “sister to archosaurs” does not mean “a living archosaur”.A large number of aligned bases is not a substitute for checking the analysis. Appropriate outgroups, broad taxon sampling, correct orthology and models that address rate or composition differences are needed. Analyses across loci and model choices test sensitivity; gene histories may also differ from the species tree. Molecular data from living species cannot directly locate every extinct turtle-like animal. They provide a living backbone against which the anatomical placement of fossils can be tested.
Stem-turtle discoveries provide a particularly discriminating anatomical test. Pappochelys, a Middle Triassic animal described by Rainer R. Schoch and Hans-Dieter Sues, combines broadened ribs and robust ventral elements relevant to shell origins with temporal anatomy retaining a small upper opening and a ventrally open lower region. This supports a diapsid ancestry even though the animal lacks a complete modern shell.[ref]
A Middle Triassic stem-turtle and the evolution of the turtle body plan by Rainer R. Schoch and Hans-Dieter Sues. Skull openings, ribs, gastralia and phylogenetic interpretation of Pappochelys
Its significance is the associated character combination, not merely a hole selected because it agrees with a molecular tree. It shows that the shell and temporal roof need not have evolved as one indivisible package.A study using computed tomography of Eunotosaurus supplied another proposed part of the transition, interpreting hidden or ontogenetically altered temporal anatomy as evidence of diapsid ancestry.[ref]
Evolutionary origin of the turtle skull by G. S. Bever and others. Computed-tomographic anatomy, ontogenetic interpretation and placement of Eunotosaurus
The proposed placement of such early forms and the biological homology of particular openings remain matters for character analysis. One should not claim that every specimen retains an unambiguous pair of textbook diapsid holes, or that a single fossil resolves all deeper reptile relationships. Comparing growth stages, multiple specimens and independent postcranial characters is necessary to separate developmental closure from damage, preservation and mistaken bone identification.The general limitation is homoplasy. Openings can expand, merge with a margin, lose separating bars or become secondarily roofed; apparently similar counts can consequently have different histories. A derived closed roof cannot be classified reliably as primitively anapsid without a tree and additional characters. Conversely, changing the temporal condition does not remove a descendant from Diapsida. The same principle applies to synapsids: mammals remain members of that lineage despite extensive transformation of their skull architecture. An anatomical grade is not automatically a clade.
Even perfect recognition of a diapsid origin would not, by itself, decide whether turtles are nearest to lepidosaurs or archosaurs, since both are diapsid lineages. Resolving that question requires informative derived characters within the radiation, rather than recounting the ancestral pair of openings. Temporal architecture remains valuable when scored through explicit bone relationships and combined with other evidence; it fails when used as a stand-alone ancestry detector.
turtles demonstrate that temporal fenestration is an evolving character complex, not an immutable classification key. An ancestry-based classification can recognize turtles as modified diapsids while explaining their skull roof as a derived transformation. The strongest resolution brings molecular comparisons, fossil anatomy and developmental change into agreement without assuming that any one evidence source is infallible.
There is no general basis for assigning behaviour a smaller causal role in macroevolution. Its immediate effects are usually easier to measure within populations, but those effects can alter lineage formation and persistence. The comparison needs a definition of “contribution”: the proportion of evolutionary changes initiated by behaviour, their magnitude, their necessity, or the strength of available evidence would give different answers. Microevolution concerns change within biological populations; macroevolution concerns patterns at and above the level of species, including speciation, adaptive radiation and extinction. They are connected processes with different objects of measurement.
At the population scale, animal behaviour changes who encounters which resources, survives, mates and reproduces. Habitat preference changes exposure to ecological natural selection; mate choice changes reproductive success; dispersal changes the spatial distribution of alleles. Behaviour can therefore affect the evolution of other traits even if the behaviour itself does not evolve. Conversely, an environmentally induced change in behaviour is not automatically evolutionary change. Learning and phenotypic plasticity can occur within one lifetime, whereas an evolutionary claim requires persistence through inherited differences or an explicitly specified process of cultural inheritance.
A simple population genetics calculation makes the distinction concrete. Let be an individual's number of copies of a focal allele, its contribution to reproduction, and . With unbiased Mendelian segregation and no other transmission change, the expected allele frequency after selection satisfies:Behaviour can change and thereby change the covariance, whether selection acts directly on a behavioural difference or on another trait whose consequences depend on behaviour. The equation does not imply that every correlation between a behaviour and reproductive success is genetic: common environment, age and condition can generate such correlations. A common garden experiment, a pedigree and measurements across environments help identify the inherited component.
Behaviour may expose a previously uncommon phenotype to selection. Foraging in a new habitat can make a different resource profitable, after which selection can refine feeding structures or behavioural response thresholds. Laboratory competitions between spadefoot tadpoles from populations differing in expression of a carnivore ecomorph found differences in resource capture and morphology consistent with adaptive refinement of a formerly plastic response. Expression without the inducing cue also supported genetic assimilation. [ref]
Plasticity-led evolution: evaluating the key prediction of frequency-dependent adaptation by Nicholas A. Levis and David W. Pfennig. laboratory competition and expression of the carnivore ecomorph in spadefoot tadpoles
This is a combination of behaviour and development, not proof that behaviour universally comes first. Genetic accommodation requires evolution of the response, rather than assuming that an acquired habit is copied directly into DNA.The opposite effect is also possible. Through phenotypic buffering, movement or flexible foraging may keep individuals in suitable conditions and reduce selection on physiological or morphological differences. Thus flexibility can promote occupation of a new environment, delay genetic divergence, or prevent local extinction. The sign depends on whether behaviour changes exposure to selection or allows animals to avoid it. A short-term adaptive response is consequently not evidence for a universal acceleration of evolutionary change.
At the boundary between populations and species, the behavioural effects are particularly direct. Assortative mating, host choice and learned signals can reduce gene flow. In the Big Bird lineage of Darwin's finches, field observations and genomic ancestry documented an immigrant Geospiza conirostris breeding with a resident Geospiza fortis and the formation of an endogamous descendant lineage. Song and distinctive morphology contributed to mating within that lineage. [ref]
Rapid hybrid speciation in Darwin's finches by Sangeet Lamichhaney and others. Science 359, pp. 224–228; immigrant ancestry, endogamy and the Big Bird lineage
The evidence links immigration, hybridization and mate recognition to rapid reproductive separation; it does not show that song alone caused isolation or establish the lineage's indefinite future persistence. Nevertheless, behaviour participates in an event conventionally classified as macroevolution.Over longer periods, these mechanisms can influence the rates of lineage origination and disappearance. Behaviour that permits colonization can expose populations to ecological opportunity and eventual adaptive radiation. Specialization in host use or mating signals can strengthen reproductive barriers. Conversely, costly reproductive competition or inflexible resource use can increase vulnerability. In fossil ostracods, greater sexual dimorphism was associated with greater estimated extinction risk, using carapace differences as a proxy for male reproductive investment. [ref]
High male sexual investment as a driver of extinction in fossil ostracods by Maria João Fernandes Martins and others. Nature 556, pp. 366–369; dimorphism as a proxy and fossil extinction estimates
This is unusually direct evidence about actual lineage loss, but an anatomical proxy does not preserve courtship or experimentally isolate sexual selection from every correlated attribute. It supports a possible connection rather than a general law that strong sexual selection causes extinction.Evaluating a claim about relative importance also requires correcting unequal evidence. Contemporary behavioural experiments can manipulate cues and follow reproduction, whereas most ancient behaviour must be inferred from traces, anatomy or living relatives. Living-only comparative studies omit extinct lineages and can confuse a trait associated with diversification with a trait that evolved after diversification. Comparisons should allow for shared ancestry, environmental opportunity and incomplete sampling, and distinguish an increased speciation rate from a reduced extinction rate. Counting observed behavioural changes over years against anatomical changes over millions of years is not a meaningful common denominator.
Behaviour has demonstrable population-level effects and plausible, sometimes well-documented effects on speciation and extinction. The stronger conclusion is that its evolutionary influence is context-dependent and transmitted across scales, while the evidence becomes harder to identify over deep time. A qualified statement about evidential accessibility is defensible; a general ranking of causal importance is not.
dispersal determines potential encounters and genetic exchange; mate preference helps determine which encounters become reproduction. speciation depends on the resulting gene flow and the evolution of barriers to it. None of the three can be understood simply from the distance animals move or from a laboratory preference score. Dispersal is movement, while gene flow requires genetic contribution to later generations. Mate preference is responsiveness to possible partners; realized mating also depends on encounter rate, competition, availability and acceptance by both sexes.
Reduced movement can allow populations to diverge through natural selection and genetic drift. During allopatric speciation, different environments, signal systems or histories can generate reproductive differences without continual exchange of alleles. At secondary contact, these differences may maintain isolation, permit extensive merging, or produce partial barriers. Current coexistence does not establish sympatric speciation: the populations may have diverged elsewhere. Conversely, appreciable movement need not prevent divergence if migrants seldom reproduce or their descendants perform poorly.
A small illustrative calculation shows why migrant numbers and effective contribution differ. Suppose migrants constitute a fraction of potential breeders, residents have reproductive weight one, and migrants have weight after mate acceptance, with equal survival and other fecundity. Their fraction of the successful breeding pool is then:For and , this is . These are invented values, not a migration estimate. The normalization matters, and the expression describes weighted breeders, not automatically ancestry in every offspring or a complete model of sex-specific mating. It nevertheless demonstrates why substantial dispersal can coexist with much smaller genetic exchange.
Movement is often nonrandom with respect to habitat. If animals select the resource on which they also meet mates, habitat preference produces assortative mating without an explicit preference for a partner's identity. In Rhagoletis pomonella, apple- and hawthorn-associated populations mate in relation to their hosts. Mark-and-recapture studies found that host fidelity substantially restricted exchange, while host preference and differences in emergence timing contributed to the barrier. [ref]
Host fidelity is an effective premating barrier between sympatric races of the apple maggot fly by Jeffrey L. Feder and others. PNAS 91, pp. 7990–7994; three mark-and-recapture studies and host-associated gene flow
The estimated exchange was not zero: the example concerns partial, measurable premating isolation, rather than complete reproductive closure. It also warns against equating geographic overlap of host plants with random encounters among insects.Ecological specialization and mating can remain coupled when the same characteristic affects both, a magic trait, or when separate relevant loci are genetically linked. Pea-aphid mapping linked host-related adaptation and reproductive isolation, making Acyrthosiphon pisum an example in which host association has a genetic basis rather than being inferred solely from field distribution. [ref]
Genetic linkage of ecological specialization and reproductive isolation in pea aphids by David J. Hawthorne and others. Nature 412, pp. 904–907; mapping host adaptation and habitat preference
A mapped association does not establish one causal mutation with several effects. Pleiotropy, tight genetic linkage and correlated environmental responses can produce similar phenotypic patterns and require different tests.Direct preference for a signal creates another route. In Heliconius, wing patterns are involved in ecological interactions and mate recognition. Genetic crosses between Heliconius melpomene and Heliconius cydno mapped major effects on male courtship preference, including a region tightly linked to the colour-pattern locus Optix. [ref]
Genetic dissection of assortative mating behavior by Richard M. Merrill and others. PLoS Biology 17, e2005902; preference QTLs, linkage to optix, and limitations of courtship assays
Such coupling helps preserve associations between cues and preferences against genetic recombination. Yet the mapping interval is not an identified “speciation gene”, and a male's courtship duration can also depend on a female's response. Manipulated or artificial models, standardized females and reciprocal behavioural assays help separate visual preference from other interacting traits. Both sexes can exert choice; a female-choice-only account would miss this example.The sensory environment can itself connect habitat and mate preference. Lake Victoria cichlids show associations among depth-related light conditions, visual-pigment variation, male colours and female preferences consistent with sensory drive. [ref]
Speciation through sensory drive in cichlid fish by Ole Seehausen and others. Nature 455, pp. 620–626; light gradients, visual pigments, colours and preferences
Preference need not begin as a direct mechanism to avoid hybrids: sensory adaptation for detecting resources can change the attractiveness of a mating signal. Changing the light environment can then weaken a previously effective colour barrier. Sensory sensitivity, signal appearance and preference are related measurements, however, and none should be substituted for an actual assay of mating or genetic exchange.Dispersal can also create rather than dissolve reproductive novelty. Founders bring new combinations of signals and developmental backgrounds into contact, and hybridization can generate a distinct combination rather than merely homogenize populations. Alternatively, repeated immigration can swamp locally favoured alleles or continually break associations between signal and preference. The outcome depends on ecological selection, the genetic architecture of the barriers, recombination, density and mating costs, not on a universal migration threshold.
After contact, reinforcement can strengthen premating isolation if hybridization imposes a fitness cost and heritable mate discrimination reduces that cost. It requires selection against the consequences of interpopulation mating, not just a finding that sympatric individuals prefer their own type. Differences between contact and non-contact populations could instead reflect habitat, population history or differential survival. Common rearing, reciprocal crosses, controlled cue presentation and direct estimates of hybrid performance make the alternatives distinguishable. Migration can supply variation needed for such evolution while also eroding the resulting barrier.
The most informative research therefore measures the entire sequence: departure, movement, settlement, encounter, mating and descendant contribution. Tracking and mark–recapture reveal movement; choice and no-choice tests reveal different aspects of preference and acceptance; parentage and genomic ancestry reveal realized reproduction. A preference assay needs controls for condition, familiarity, developmental experience and stimulus intensity. Barriers operating at successive stages must be assessed conditionally, rather than adding percentage reductions that refer to different denominators. speciation becomes possible when ecological and mating processes maintain sufficiently persistent reproductive separation; dispersal and mate preference jointly determine that separation and can either strengthen or weaken it.
Sensory genetics shows that evolution can change receptor molecules, their expression and neural organization, and that the relation between genes and perception is neither one-to-one nor confined to protein-coding mutations. Genetic architecture concerns the number, effects, interactions and arrangement of contributing variants in a specified population and environment. Identifying a receptor is one achievement; explaining variation in sensory performance, its development and its evolutionary consequences requires several additional steps.
A foundational result is that a large sensory repertoire can arise by gene duplication followed by divergence. Cloning of human visual-pigment genes revealed related but distinct short-, medium- and long-wavelength-sensitive pigments, with particularly close sequence similarity between the latter two. [ref]
Molecular genetics of human color vision: the genes encoding blue, green, and red pigments by Jeremy Nathans and others. Science 232, pp. 193–202; cloned visual-pigment genes and sequence comparisons
This links colour vision to a history of related opsins, rather than requiring a wholly new biochemical mechanism for every sensitivity. However, additional gene copies need not produce additional functional sensory channels: copies can be lost, expressed together, or differ too little in sensitivity to support useful discrimination.The distinction follows from the physics of receptor stimulation. In a simplified model, input to receptor class is proportional to:where is the light spectrum reaching the eye and its effective spectral sensitivity. Different spectra can produce the same , so a single receptor cannot independently determine wavelength and intensity. Comparing multiple receptor classes allows more information, but the animal also needs suitable neural circuits, a decision process and an appropriate task. Thus an opsin sequence is not a complete description of a perceived colour, and a colour vision test must vary brightness to prevent intensity from supplying the answer.
Regulatory differences can be as important as changes in the receptor sequence. Crosses between cichlid species expressing different opsin combinations identified relatively few regions contributing to expression differences, including both cis-regulatory elements and trans-regulation. [ref]
Genetic basis of differential opsin gene expression in cichlid fishes by Karen L. Carleton and others. Journal of Evolutionary Biology 23, pp. 840–853; crosses and cis- and trans-acting regulatory regions
The same inherited receptor repertoire can therefore support different visual sensitivities through deployment of different members. A trans-acting regulator can coordinate several genes, whereas a local regulatory change can alter a more restricted expression pattern. These are mechanistic possibilities, not a rule that cis changes are always specific or trans changes always costly. Developmental stage and light exposure also matter, so comparisons need common rearing, matched ages and measurements beyond a single transcript sample.Experimental addition of a receptor can test whether downstream processing can use the new input. Adding a human long-wavelength opsin to adult dichromatic Saimiri sciureus produced new colour-discrimination performance. [ref]
Gene therapy for red-green colour blindness in adult primates by Katherine Mancuso and others. Nature 461, pp. 784–787; adult squirrel monkeys, added L opsin and colour discrimination
The result challenges the assumption that a new sensory channel always requires a matching circuit assembled only in early development. It does not imply that every sensory deficit can be corrected this way or that the monkeys' subjective experience became identical to a human's. Stable pre-intervention performance, tests across chromatic directions and controls against brightness cues make the inference stronger than expression of the introduced gene alone.Olfaction reveals a related architecture at a larger receptor repertoire. Molecular cloning identified a very large family of candidate olfactory receptor genes with expression in olfactory tissue. [ref]
A novel multigene family may encode odorant receptors: a molecular basis for odor recognition by Linda B. Buck and others. Cell 65, pp. 175–187; cloning a large receptor gene family from olfactory tissue
This supplies diversity of molecular recognition, but it does not imply one gene for every odour or one receptor for every behavioural response. Odour mixtures and concentrations can engage overlapping inputs, and the same sensory input can acquire different significance through context and learning. Establishing receptor function requires physiological responses to defined stimuli, appropriate expression controls and comparison with cells lacking the receptor.genes also help organize the neural map receiving those inputs. Labelling mouse neurons expressing a particular receptor showed convergence at characteristic locations in the olfactory bulb. Receptor-swap experiments changed targeting, indicating a contribution of receptor identity to axon guidance. [ref]
Visualizing an Olfactory Sensory Map by Peter Mombaerts and others. Cell 87, pp. 675–686; labelled receptor-expressing neurons and receptor-swap experiments
The receptor was not the sole determinant: the resulting projection was not simply an arbitrary map wholly specified by the substituted molecule. This connects molecular recognition with neural development and illustrates pleiotropy, while leaving room for other guidance mechanisms and activity-dependent refinement. A gene can influence the wiring through which its own sensory signal will be interpreted.Sensory loss likewise need not mean simple destruction of a receptor gene. In cave populations of Astyanax mexicanus, increased embryonic Hedgehog signalling was associated with lens apoptosis and arrested eye development; experimental overexpression in surface fish reproduced important elements of the phenotype. [ref]
Hedgehog signalling controls eye degeneration in blind cavefish by Yoshiyuki Yamamoto and others. Nature 431, pp. 844–847; midline expression, lens apoptosis and experimental overexpression
Manipulating a developmental pathway therefore provides causal evidence beyond observing an association between cave residence and blindness. It does not identify every naturally selected causal variant, prove that eye reduction was directly favoured rather than indirectly associated with other traits, or establish the same mechanism in all cave populations. Developmental competence and the adult phenotype can differ substantially.These findings also connect sensory genetics with speciation. In Lake Victoria cichlids, differences in the light environment, visual pigments, mating signals and preference were associated with reproductive differentiation. [ref]
Speciation through sensory drive in cichlid fish by Ole Seehausen and others. Nature 455, pp. 620–626; light gradients, visual pigments, colours and preferences
The connection is that selection on obtaining information can change the relative effectiveness of signals; it is not a claim that every opsin variant is an isolating barrier. One must separately establish expression, sensitivity, preference and reproductive consequences.Several general methodological lessons follow. A quantitative trait locus is an interval associated with variation, not automatically the causal gene. A large detected effect does not exclude many small effects, and laboratory crosses may sample only a subset of natural variants. Fine mapping, allele replacement, reciprocal genetic backgrounds, a genetic rescue experiment and neural or behavioural measurements can connect successive causal steps. Pleiotropy, genetic linkage and environmental covariance require different explanations even when all produce correlated sensory traits. Conversely, absence of segregating variation in one laboratory stock says little about all evolutionary routes available to a lineage.
Sensory systems can evolve through changes in molecular recognition, gene regulation, developmental organization and use of existing circuitry. Their genetic architecture both enables and constrains these routes, while functional experiments are needed to connect a genomic difference to an animal's sensory performance.
Lack of direct access to another animal's subjective experience limits some claims about consciousness, but does not prevent testable explanations of sensory processing, behavioural function or evolutionary history. The essential distinction is between occupying another individual's standpoint and explaining what information it acquires, how it uses that information, and the consequences for survival and reproduction. Thomas Nagel's argument concerns the subjective character of experience, rather than a claim that objective bat biology is inaccessible. [ref]
What Is It Like to Be a Bat? by Thomas Nagel. The Philosophical Review 83, pp. 435–450, especially pp. 439–442: subjective standpoint versus objective description
For behavioural biology, Tinbergen's four questions keep the explanatory targets separate. Mechanism asks what sensory and neural processes produce a response; development asks how it changes with maturation and experience; function asks how it affects performance or fitness; evolutionary history asks how it arose and differs among relatives. [ref]
On aims and methods of Ethology by Nikolaas Tinbergen. Zeitschrift für Tierpsychologie 20, pp. 410–433; causation, development, survival value and evolution
Not knowing a bat's exact experience does not make the latter questions equivalent to guessing its feelings. It does mean that a functional explanation, even a very successful one, is not by itself an explanation of the qualitative character of consciousness.Echolocation illustrates substantial knowledge without shared phenomenology. Acoustic recordings and experiments on sensory access linked ultrasonic vocalization and hearing to obstacle avoidance in flying bats. [ref]
The sensory basis of obstacle avoidance by flying bats by Donald R. Griffin and others. Journal of Experimental Zoology 86, pp. 481–506; acoustic and sensory tests of obstacle avoidance
Modern tests can vary echo delay, level or interference while measuring detection or flight responses. A prediction about ranging is available from propagation physics: for sound speed , a round-trip echo delay from a stationary target at distance gives approximately:An illustrative delay at corresponds to . The factor two comes from outward and return travel. Real ranging also depends on target motion, atmospheric conditions, filtering and the timing of emission. None of these testable relationships requires a scientist to experience an echo as the bat does.The experimental controls matter because a successful animal can exploit an unintended cue. Changing a visual target might also change its acoustic reflection; changing an echo's delay might accidentally change its intensity. Appropriate comparisons manipulate the putative information while holding other cues constant, include sham manipulation, and measure baseline performance. A psychometric function across stimulus levels is more informative than a single success rate. Signal detection theory distinguishes sensitivity from response criterion, helping separate a sensory change from greater willingness to respond. Failure in an unfamiliar apparatus may reflect motivation or the required motor response rather than absence of the sensory capacity.
This approach also prevents treating human perception as the definition of available information. A stimulus invisible to us or outside our hearing range can be salient to the animal. The correct physical description must use the animal's receptors, spatial and temporal resolution, and ecological setting. Human photographs, displays and loudspeakers can omit relevant information or introduce artefacts. Conversely, an animal's failure to categorize objects in our preferred way need not show poor understanding: the experimental categories may not correspond to the distinctions its biology makes useful. Sensory ecology is therefore a substantive constraint on design, even though the animal's qualitative viewpoint remains partly inaccessible.
Causal intervention can connect sensory machinery to behaviour without settling phenomenology. The adult squirrel-monkey opsin-addition experiment demonstrated improved chromatic discrimination following a specified alteration of receptor input. [ref]
Gene therapy for red-green colour blindness in adult primates by Katherine Mancuso and others. Nature 461, pp. 784–787; adult squirrel monkeys, added L opsin and colour discrimination
That supports a functional inference about information use. It cannot report the appearance of the new colours to a monkey. Distinguishing these claims makes the experiment more, rather than less, informative: its conclusion is tied to an observable prediction instead of an assumed human-like experience.Similarly, we can study affect-like influences on decisions without claiming to have measured a feeling directly. In bumblebees, unexpected sucrose reward altered responses to ambiguous cues, with evidence for a dopamine-dependent component and tests of behaviour in more than one context. [ref]
Unexpected rewards induce dopamine-dependent positive emotion-like state changes in bumblebees by Clint J. Perry and others. Science 353, pp. 1529–1531; ambiguous-cue tests, sucrose reward and dopamine manipulation
Such judgement bias is evidence of an internal state influencing decisions; it is not a direct readout of happiness. Changes in activity, hunger, reward valuation or stimulus discrimination can produce superficially similar results and require control. Nor is an unexplained behavioural difference stronger evidence for subjective experience merely because an experimenter finds it familiar.Evolutionary explanations require an additional bridge. Showing that a bat uses echoes establishes a mechanism; showing improved capture or obstacle avoidance under relevant conditions tests a current function. Demonstrating historical adaptation additionally requires comparisons, inherited variation and an account of the selection pressures or ancestry involved. One can test the prediction that signal structure differs with clutter or prey characteristics while allowing for shared ancestry and body size. A useful hypothesis should predict differences under specified circumstances, rather than explain every outcome retrospectively by invoking what the animal “wanted”.
There are nevertheless real limits. Different internal models can generate the same choice, and an animal cannot necessarily provide the linguistic reports that make some human experiments possible. Success with one discrimination does not reveal the complete content of a representation, and a neural correlate does not uniquely specify an experience. Questions about felt intensity, emotional quality or a reflective awareness of self demand converging behavioural and physiological evidence and may remain underdetermined. This is an epistemic limitation, not evidence that the corresponding experiences are absent.
A productive position avoids both unconstrained anthropomorphism and an equally unsupported denial of mental processing. Specify which sensory information or internal state the model requires, derive predictions, test alternatives and state the level of inference. We can explain much of the evolution and function of animal behaviour through objective relationships among information, decisions and fitness, while remaining uncertain about precisely what those processes feel like to the animal. The residual uncertainty should limit the wording of our conclusions and improve experimental design, rather than stop the research.
Non-human animals show evidence for several components of social-state tracking, but the evidence does not establish a uniform, human-like theory of mind. Theory of mind should be decomposed into sensitivity to goals, visual access, knowledge and belief, rather than treated as a single ability that an animal either possesses or lacks. The central evidential question is whether behaviour requires representing another's mental state, or can be explained by learned relationships among observable actions, contexts and outcomes.
Goal attribution has support from experiments distinguishing similar outcomes produced by different actions. Chimpanzees responded differently to a person who was unwilling to transfer food and one who was willing but unable: they persisted differently and left earlier in the unwilling condition. [ref]
‘Unwilling’ versus ‘unable’: chimpanzees’ understanding of human intentional action by Josep Call and others. Developmental Science 7, pp. 488–498; matched food-withholding outcomes and differing actions
Holding the absence of food transfer broadly constant prevents the explanation that any unrewarded trial produces the same reaction. The contrast supports sensitivity to the organization or apparent purpose of actions. However, differences in movement and affect remain observable cues, so the finding need not imply a fully explicit concept of intention. Generalization to new obstacles and action sequences is a stronger test than repeating familiar signals.Visual perspective taking concerns another individual having a different view. When dominant and subordinate chimpanzees competed for food, subordinates preferentially obtained food to which they had better visual access. Giving the subordinate a headstart forced its choice before the dominant's approach could reveal the answer, reducing a straightforward movement-following explanation. [ref]
Chimpanzees know what conspecifics do and do not see by Brian Hare and others. Animal Behaviour 59, pp. 771–785; occlusion, competitive food choice and subordinate headstart controls
Such controls support tracking of another's visual access. They do not show that the subject represents every aspect of how the scene looks to the other animal; access to an object is a narrower problem than its appearance from a different viewpoint.The distinction extends from seeing to knowing. An animal can potentially remember whether another witnessed hiding even after neither currently sees the food. Controlled competitive tasks found chimpanzees sensitive to knowledge versus ignorance, yet not successful in closely related false-belief conditions. [ref]
Chimpanzees know what others know, but not what they believe by Juliane Kaminski and others. Cognition 109, pp. 224–234; matched knowledge–ignorance and false-belief competition tests
Knowledge attribution therefore has stronger support in those tasks than an unrestricted ability to predict action from mistaken beliefs. Negative performance is not proof of incapacity: memory, inhibitory demands, motivation and task comprehension may limit the response. But a positive result for knowledge should not be relabelled a positive result for belief simply because both are social.Bird studies provide evidence beyond primates. Ravens that had experienced a peephole altered cache-protection behaviour when a potential observer could be heard but not seen. The use of recorded sounds removed an actual competitor's gaze and movements as immediate guides, and the manipulation of available visual access made the test more informative than comparison of merely occupied and empty rooms. [ref]
Ravens attribute visual access to unseen competitors by Thomas Bugnyar and others. Nature Communications 7, 10506; peephole experience, playback and caching in the absence of visible competitors
This supports generalization from access conditions to a possible observer. It remains possible to model performance through learned relations between openings, sounds and risk; novel transfer tests are needed to distinguish how abstractly the bird represents “being seen”.Experience with one's own actions can also change responses to others. Scrub jays with previous pilfering experience showed stronger re-caching responses after having been observed caching. [ref]
Effects of experience and social context on prospective caching strategies by scrub jays by Nathan J. Emery and others. Nature 414, pp. 443–446; prior pilfering experience and re-caching after observation
One interpretation is projection of the bird's own pilfering experience onto a potential competitor. Another is acquisition of a more general rule about cache vulnerability. The finding makes prior experience a causal candidate and suggests a relation between self and other, but it does not establish that the bird consciously imagines another individual's intentions. Observed and unobserved caching, prior experience and the opportunity to relocate food all need to be distinguished.False-belief understanding sets a particularly demanding criterion: the subject must predict an agent using information that the subject knows is wrong. In great apes, an anticipatory looking paradigm found looks towards the location where an agent falsely believed an object remained, even when the subject had seen the object's removal. [ref]
Great apes anticipate that other individuals will act according to false beliefs by Christopher Krupenye and others. Science 354, pp. 110–114; anticipatory looking in false-belief scenarios
This bypasses some demands of an active food-choice response. Yet gaze towards a previously attended location can also arise from action prediction, attentional cues or associations with where an actor last saw an object. Anticipation is therefore evidence about prediction, whose representational basis needs further controls.A subsequent experiment manipulated the ape's own experience of a barrier that looked the same from a distance but was either opaque or translucent. All subjects then watched the same test actions. Those with the opaque experience were more likely to anticipate the actor searching according to the outdated location. [ref]
Great apes use self-experience to anticipate an agent’s action in a false-belief test by Fumihiro Kano and others. PNAS 116, pp. 20904–20909; visually matched opaque and translucent barriers and identical test videos
Because the visible test behaviour was held constant, an explanation relying only on a difference in the actor's immediate behaviour was weakened. The result supports transfer from self-experience to another's informational situation. It still leaves questions about the breadth of the represented belief: a limited model of visual registration and action expectation may succeed without the flexible propositional reasoning characteristic of human language.Taken together, positive anticipatory-looking results and negative active-choice results need not be forced into a single yes/no answer. The tasks measure different outputs and impose different demands. Stronger evidence would show the same individuals generalizing across novel agents, objects and routes of access, distinguishing true belief, false belief and ignorance while physical events, attention and rewards are controlled. Eye-tracking analyses should specify regions and timing in advance, report the subjects who produce no usable anticipatory look, and avoid inferring population-wide competence solely from a selected subset of trials. Replication and uncertainty around effects matter especially with small captive samples.
The relation to self-representation is similarly componential. Using one's experience of a transparent barrier to predict another's access suggests some correspondence between self and other. It does not demonstrate an autobiographical self or reflection on one's own beliefs. Metacognition, such as selective information seeking when knowledge is missing, concerns monitoring one's own processing and is not equivalent to attributing knowledge to somebody else. Mirror self-recognition concerns one's body and is neither a necessary consequence nor a sufficient demonstration of belief attribution. These distinctions prevent a visually based test from becoming a universal scale of mentality.
The defensible conclusion is a mosaic: animals can track goals and access, some experiments support knowledge attribution and belief-sensitive predictions, and the most elaborate interpretation remains contested. The experiments constrain possible representations of self and others; their value lies in progressively excluding alternatives, rather than naming a mental state after any apparently intelligent social response.
I would combine quantitative-genetic cross-fostering with controlled transfer of maternal brood-chamber material in the dung beetle Onthophagus taurus. The hypothesis is that maternal genetic differences influence offspring development partly through the amount of food provided and partly through the composition of material transferred from the mother's body. These pathways must be separated: a larger brood provision, a beneficial microorganism and an inherited offspring allele can all increase offspring mass, but imply different mechanisms.
The system has three relevant precedents. A paternal half-sib study of Onthophagus taurus detected genetic variation in maternal brood provisioning and substantial maternal contributions to offspring phenotype. [ref]
The genetics of maternal care: direct and indirect genetic effects on phenotype in the dung beetle Onthophagus taurus by John Hunt and others. PNAS 99, pp. 6828–6832; paternal half-sib design, brood mass and maternal contributions
A separate study reared this species with sterile dung and detected maternal contributions and shared bacterial sequences in the brood chamber and offspring, supporting transmission through the provisioned environment. [ref]Brood ball-mediated transmission of microbiome members in the dung beetle, Onthophagus taurus (Coleoptera: Scarabaeidae) by Anne M. Estes and others. PLoS ONE 8, e79061; sterile dung, brood-chamber material and parent–offspring bacterial sequence comparisons
Experimental developmental benefits of pedestal-associated microbiota were demonstrated in Onthophagus gazella, including context dependence under environmental stress; those functional results should not be assumed automatically to hold in Onthophagus taurus. [ref]Developmental and Ecological Benefits of the Maternally Transmitted Microbiota in a Dung Beetle by Daniel B. Schwab and others. The American Naturalist 188, pp. 679–692; Onthophagus gazella, pedestal removal and environmental stress
The conceptual link is an indirect genetic effect: the provider's genotype affects the recipient's phenotype through a rearing environment. The transferred mediator would be maternal faecal or secreted material, including associated viable microorganisms and soluble products. This fits the socially transferred material framework because the mother contributes material processed in or produced by her body; collecting external dung alone would not establish such a transfer. [ref]
Socially transferred materials: why and how to study them by Sanja Maria Hakala and others. Trends in Ecology & Evolution 38, pp. 446–458; framework and distinction from merely collecting external food
The actual molecular mediator is an experimental question. Finding bacterial DNA or a protein in a brood chamber does not establish that it is alive, active, beneficial, or responsible for an indirect genetic effect.First establish a common-garden breeding population with a recorded pedigree and genotype markers. Use a paternal half-sib design with several dams per sire and several adult daughter providers per dam, distributed among independently randomized rearing containers. Standardize donor age, mating history, developmental nutrition and adult diet, and block dung source, moisture and temperature. Because maternally inherited microbes can themselves produce family resemblance, rear replicate provider families with a standardized microbial inoculum in an additional common-rearing arm. Persistence of a family difference alone is insufficient evidence for host genetic causation.
For the initial cross-fostering experiment, allow each provider to construct several brood balls on weighed, standardized dung. Measure construction time, final dry-mass estimate from matched material, egg-chamber properties and maternal faecal pedestal quantity. Remove the original egg before hatching and replace it with an age-matched egg from a separately bred recipient family. Randomize recipient families across provider families, with reciprocal assignments and repeated providers; include handled own-egg and untouched controls. Record egg size and biological-mother identity so that egg provisioning and other pre-transfer maternal effects are not silently attributed to the foster provider.
One possible balanced allocation has 20 sire families, two dams per sire and two daughter providers per dam, giving 80 providers. Four independently prepared brood balls per provider yield 320 offspring-rearing units, allocated across multiple recipient families and collection blocks. This is an illustrative feasible structure, not a claim of adequate power. The effective replication for a sire-level genetic component is much smaller than 320; repeated balls estimate provider consistency and within-provider variation. A pilot-based simulation of the planned pedigree, variance components, mortality and missing samples should determine the final scale before outcomes are examined.
Measure larval growth trajectories, survival, development time and adult size; subsequently measure reproductive performance where feasible. Score provisioning behaviour blind to family and recipient treatment. Collect matched donor and provision samples for absolute microbial load, community composition and soluble chemical profiles. Include extraction blanks, reagent controls and bacterial-load standards, especially because low-biomass sequence samples are vulnerable to contamination. Shared 16S sequences provide limited discrimination among strains; culture or higher-resolution sequencing can test whether a donor-associated strain actually reaches and persists in a recipient.
For an offspring reared in a ball prepared by provider , an animal model in quantitative genetics could use:Here is the direct genetic effect of the offspring, the additive provider contribution, a repeatable non-genetic provider effect, a biological-mother effect, and prespecified batch and rearing terms. Genetic effects use the pedigree or genomic relationship matrix; provider identity alone cannot identify . If the pedigree contains informative relatives in both roles, direct–indirect genetic covariance can also be estimated. Otherwise that covariance is not identified by the first experiment and should not be assumed known. Crossed recipient and provider families distinguish a general provider effect from matching between a particular recipient genotype and provider background.
The second experiment tests the transferred pathway rather than merely adding a microbial measurement to that model. Construct uniform artificial brood balls with the same treated dung, food mass and chamber geometry, and transfer equal donor-equivalent pedestal material. Compare intact material, material separated into a cell-free soluble fraction, a preparation containing non-viable microbial cells, and a live-cell add-back or rescue preparation. Include material-free, medium and sham-processing controls, together with untreated natural balls as a benchmark. Test viability rather than inferring it from a sterilization label. All processed-dung groups must share the same processing, because sterilization can also change nutritional and chemical properties.
Within a subset, exchange washed live-cell fractions and soluble fractions independently between donor families. A crossed donor-cell-source by donor-soluble-source design asks whether offspring differences track microbial cells, soluble maternal products, or their interaction. Hold total food quantity and transfer volume constant. Include both a standardized live-cell dose, testing compositional differences, and a naturally varying dose arm, testing a possible maternal-genotype effect on delivered quantity. An equal-dose experiment alone could erase a real dose-mediated pathway. Test a candidate cultured community or identified molecule in a dose range anchored to measured natural transfers, rather than interpreting a large artificial supplement as evidence for normal function.
The predicted pattern is specific. If food mass explains the provider effect, equalizing mass should greatly reduce it. If viable maternal microbes mediate an additional effect, removing viability at equal food quantity should reduce the relevant donor-associated growth difference, and a compatible live add-back should restore it. An effect retained in a cell-free fraction instead motivates identifying soluble maternal or microbial products. A failed rescue can reflect processing damage or a missing microbial partner, rather than absence of any natural pathway. If all provider differences disappear after standardized rearing, a non-genetic maternal or microbial inheritance explanation becomes more plausible than the proposed host genetic effect.
Analyse the cross-fostering data first for total provider genetic contributions, then analyse the randomized material manipulations for mechanism. Simply adjusting for a measured mediator can block part of the effect or introduce bias; causal mediation needs assumptions and experimental support. Prespecify the primary outcomes, appropriate survival analysis, family and donor clustering, planned contrasts and treatment-by-recipient-background interactions. Offspring within a maternal pedigree and repeated chemical measurements are not independent genetic replicates. Measure provider costs, such as future fecundity and provisioning effort, because faster-growing offspring alone do not establish the evolutionary advantage of the provisioning behaviour.
The decisive result would connect provider genotype to a measured transfer difference and then experimentally connect that difference to recipient performance, independently of offspring genotype and food quantity. Negative outcomes remain informative: maternal influence without additive provider variance is a maternal effect without the demonstrated genetic component, while heritable provisioning effects without a material-mediated mechanism leave a genuine indirect genetic effect whose pathway is still unresolved.
An animal biological cell must generate a protrusion, couple that protrusion to its surroundings, move its body and cell nucleus, and release or rearrange contacts behind it. Cell polarity makes these events persistent in one direction. At cellular scales, inertia is usually negligible: active forces balance resistance continuously, rather than giving the cell momentum that carries it forward after propulsion stops. ATP consumption maintains the system away from thermodynamic equilibrium.
At the front, actin polymerization can push the cell membrane into a lamellipodium. Whether this produces advance depends on coupling to the environment: without a mechanical grip, the actin network can move backward instead. On a flat adhesive substrate, integrins bind the extracellular matrix and connect through focal adhesions to the cytoskeleton. Regulated engagement transmits traction, while rearward myosin contraction and adhesion turnover move the rest of the cell. Adhesions must resist slipping long enough to transmit force but release to avoid anchoring the rear indefinitely. Another protrusive mechanism is a membrane bleb: local separation of the cell membrane from the cell cortex, driven by intracellular pressure, expands the membrane before a new cortex assembles underneath it.
A two-dimensional culture surface offers a broad basal contact area and little geometrical obstruction above the cell. A three-dimensional environment adds pore size, fibre orientation, matrix stiffness, and resistance from surrounding cells. The same cells may switch between elongated, strongly adhesive migration and more rounded, weakly adhesive movement. Proteolysis can enlarge a path through the extracellular matrix, but a sufficiently permissive existing pore need not require digestion. The relatively stiff cell nucleus can become the main bottleneck; its passage depends on deformation, confinement and force transmission. Extensive squeezing can damage the nuclear envelope, so migration speed alone is not a sufficient measure of successful transit.
A decisive experiment removed all functional integrins from mouse leukocytes. Their interstitial migration in three-dimensional environments persisted, and myosin became particularly important for passage through narrow gaps. This distinguishes force generation from a particular adhesion mechanism: confinement and friction can provide useful coupling even without integrin anchoring.[ref]
Thus “three-dimensional migration requires stronger adhesion” is not a general rule. A useful comparison holds ligand density, matrix stiffness and pore geometry as independently controlled as possible, measures whole-cell and nuclear movement, and perturbs actin, myosin, integrins and matrix digestion separately. Differences then identify which mechanical requirement has changed, rather than treating dimensionality as a single unexplained variable.
The hypothesis has two distinct components: the tissue changes its material response, and that change causally affects collective cell migration. A moving tissue may generate different stresses without becoming mechanically different. Conversely, a changed viscosity or yield stress need not generate directed movement without a driving force. The experiment should distinguish force production, material response and geometry.
First obtain a time-resolved three-dimensional map of the embryo using minimally perturbing live-cell imaging. Label nuclei and membranes, register tissue motion, and measure cell speeds, directional persistence, neighbour exchanges, strain rates and the timing of morphogenesis. Track cells relative to their neighbours as well as to the microscope: bulk translation alone does not show internal rearrangement. Compare equivalent developmental stages and anatomical regions, and quantify cell proliferation, death and differentiation so that changes in tissue composition are not mistaken for migration.
Next apply a calibrated mechanical perturbation. An embedded deformable droplet with known interfacial properties can report anisotropic stresses; magnetic actuation can impose a controlled deformation and reveal recovery, viscoelasticity and a possible yield stress. A controlled force step followed by relaxation probes different timescales. Laser ablation of a loaded junction provides a complementary recoil measurement, but recoil velocity depends on both pre-existing tension and dissipation: it is not an absolute tension measurement without a mechanical model. Probe different directions because tissue response may be anisotropic.
An informative precedent combined magnetically actuated droplets and cell tracking in the extending zebrafish body axis. Posterior tissue was more fluid-like than the more mature anterior region. Perturbations of N-cadherin and contractility helped connect adhesion and rearrangements to mechanical integrity and elongation.[ref]
A fluid-to-solid jamming transition underlies vertebrate body axis elongation by Alessandro Mongera and others. Figures 1–3, droplet-based stress/yield measurements and cell rearrangements; Figure 4, relation to axis extension
This motivates a specific mechanism to test in the new embryo; it does not establish that all migrating tissues undergo the same transition.For causality, change the proposed material property locally and acutely, before migration changes. For example, use optogenetics to alter contractility in a defined region, or a reversible adhesion perturbation, with unilluminated and light-only controls. Measure the material response again rather than assuming the manipulation made the tissue stiffer. Then test whether the spatial pattern and timescale of migration change as predicted. Restore the perturbed component or reverse the manipulation to seek rescue. Mosaic interventions help distinguish changes in migrating cells from changes in their surroundings, although altered signal transduction remains a potential confounder.
Finally fit a mechanical model to measured stresses, geometry and material parameters, then predict a held-out perturbation rather than merely fitting the original flow. Replicate across embryos, randomize treatment, analyse trajectories blind to treatment, and use the embryo as the independent biological replicate. Evidence is strongest when a measured material change precedes movement, targeted intervention changes both in the predicted way, and rescue restores both without simply restoring tissue viability.
External chemical signals can guide cell migration, but the statement is too strong if “determined” means that they uniquely specify whether, how fast and in which direction a cell moves. A chemoattractant gradient biases a cell's internal polarity machinery; it does not directly supply the mechanical work of locomotion. Chemotaxis is directional bias, whereas a change in speed or persistence without directional preference is chemokinesis.
A chemical response depends on receptor abundance, signalling adaptation and the cell's existing cell polarity. The same external field can therefore yield different trajectories in different cell states. Uniform stimulation can increase motility without providing a direction, and spontaneous fluctuations of the actin system can initiate movement without a spatial chemical instruction. Persistent migration combines feedback within the cell with a cue that biases that feedback.
Mechanical and geometrical inputs also matter. Durotaxis describes a bias associated with substrate stiffness, while haptotaxis follows spatial variation in adhesive ligands. Contact guidance by fibre alignment can channel motion even when soluble signals are uniform. Narrow spaces constrain the available paths and can force a switch of protrusive mechanism. These effects are not wholly separate from chemistry: cells sense mechanical forces through molecular interactions. Nevertheless, their directional information resides in mechanics or geometry, not necessarily in an imposed soluble concentration gradient.
Contacts between cells supply another source of organization. Experiments on neural crest cells showed that collisions can cause protrusion collapse and repolarization, and that perturbing noncanonical Wnt signalling disrupts this behaviour and group directionality.[ref]
Contact inhibition of locomotion in vivo controls neural crest directional migration by Carlos Carmona-Fontaine and others. Collision assays in vivo and in vitro; perturbation of noncanonical Wnt signalling and local RhoA activation
Contact inhibition of locomotion therefore helps generate collective trajectories through local interactions, rather than each cell independently reading a complete external chemical map. Cohesion and other attractive interactions can prevent such repulsion from simply dispersing the group.A discriminating experiment independently varies soluble gradient, adhesive pattern and mechanical confinement. Measure direction, speed and persistence separately; reverse the gradient, remove it, and then block the relevant receptor while checking viability and the ability to move. If a directional bias follows the reversed chemical field, that supports chemical guidance. If speed rises under uniform stimulation, that supports chemokinesis. If trajectories remain aligned with fibres after chemical reversal, physical guidance is influential. Manipulating intracellular polarity can test whether a cue is instructive or merely permissive.
The useful conclusion is that motion emerges from an internally powered, state-dependent cell interacting with chemical, mechanical and cellular surroundings. External chemical signals are often decisive inputs, but the trajectory is a property of the coupled system.
A good in-vitro model should distinguish cancer invasion, movement across a tissue boundary into surrounding material, from simple growth or movement across a flat surface. No single assay reproduces the entire sequence from a primary tumour to a distant metastasis. Choose the assay to answer a specified mechanistic question, then confirm the result in a model that retains additional biological constraints.
A scratch assay measures closure of a gap in a monolayer. It is inexpensive and permits live-cell imaging, but closure combines cell migration, spreading and cell proliferation, and the wound releases signals and damages cells. It does not by itself demonstrate invasion through a basement membrane. A porous-membrane assay can measure transit toward a stimulus; adding an extracellular barrier tests an additional requirement. Yet pore size, coating thickness, chemical gradients and the counting time can dominate the result, and endpoint cell counts hide whether treatment altered survival or actual migration.
Three-dimensional tumour spheroids or organoids embedded in a defined extracellular matrix allow individual and collective invasion to be followed over time. Quantify invasion distance, cell escape, strand architecture and leader-follower behaviour, alongside changes in spheroid size and viability. Use collagen-rich and basement-membrane-like environments to test whether a phenotype depends on matrix identity. Independently vary ligand presentation, matrix stiffness and pore dimensions where possible: increasing collagen concentration changes several of them simultaneously.
A primary study of breast tumour organoids identified invasive leader cells expressing a basal epithelial programme, including K14 and p63; reducing either component impaired collective invasion in that system. The experiment connected a defined cellular subpopulation to an invasion phenotype rather than assuming that every tumour cell was equivalent.[ref]
Collective invasion in breast cancer requires a conserved basal epithelial program by Kevin J. Cheung and others. Three-dimensional organoid invasion assays; K14/p63 leader-cell observations and knockdown tests
Its conclusion remains specific to the tested settings and does not make these markers universal requirements for invasion.Add stromal cells, immune cells or a vessel-like boundary if the question concerns their interactions. Microfluidics can impose controlled gradients and permit live-cell imaging of entry into or exit from a channel. Include non-invasive and invasive controls, perturbation controls, rescue where feasible, and matched measurements of cell proliferation and death. Follow individual cells rather than relying solely on a final stained area. Patient-derived material should include multiple independent tumours: many fields from one culture are not independent patient replicates.
Limitations remain substantial. Culture selects cells that tolerate the medium; long-passaged lines may lose the original tumour's diversity. Matrices and added growth factors can have variable composition. Isolated cultures omit native immune surveillance, vascular perfusion, whole-organ architecture and systemic influences. Even elaborate organoids incompletely reproduce these features. Finally, invasion is only one stage: it does not establish survival in blood, colonization of a distant organ, or clinical response. Agreement across complementary assays strengthens a mechanism; no dish-based result alone proves a metastatic outcome in a person.
The robust starting point is a topological accounting problem. An archaeal host related to Asgard archaea and an Alphaproteobacteria-related partner must become a cell with an internal mitochondrion, a cell nucleus separated from the cytoplasm, and an interconnected endomembrane system. Their modern relatives are not unchanged ancestors. Several historical sequences can satisfy these endpoints, so the required transformations should be separated from one particular engulfment story.
The bacterial partner must become enclosed within the host's overall cellular boundary and maintained through host reproduction. Its descendants retain inner and outer mitochondrial membranes, requiring preservation or remodelling of ancestral bacterial envelope topology rather than fusion of every membrane into one. If entry used engulfment, host membrane extension, closure and a fission event would enclose the partner, and an additional host-derived surrounding membrane would have to be removed or incorporated into the evolving system. If protrusions grew around an external partner and fused, an alternative sequence could internalize it without a fully developed modern phagocytosis pathway. The modern mitochondrial envelope alone does not decide between these routes.
The host also needs a plasma membrane separating its final cytoplasm from the environment. Producing internal compartments requires membrane curvature, membrane growth and controlled membrane fusion or membrane fission. A purely continuous infolding of the surface has an extracellular-facing lumen; invagination changes geometry but does not allow a molecule to cross a lipid bilayer. Subsequent sealing and traffic can produce an internal lumen while preserving this orientation. This distinction is developed under topology of membrane compartments.
For the cell nucleus, two membranes surround the chromosome-containing compartment, with the outer nuclear envelope continuous with the endoplasmic reticulum. Openings through the envelope become selective nuclear pore complexes, while the chromosome compartment must communicate with the cytoplasm for transport without losing its identity. In an outside-in scenario, internal membranes expand around the chromosomes and fuse. In an inside-out scenario, protrusions from an ancestral chromosome-containing body expand and merge into a surrounding cytoplasm; the original boundary contributes to the nuclear boundary. The latter is an explicit alternative hypothesis, not an observed reconstruction of the event.[ref]
An inside-out origin for the eukaryotic cell by David A. Baum and Buzz Baum. Proposed sequence of protrusion growth, fusion and formation of the nuclear/ER topology
Culturing an Asgard archaeon revealed extensive protrusions and close metabolic associations, motivating an entangle–engulf–endogenize proposal. The culture was not observed making a eukaryotic cell or engulfing a bacterium, and it lacked the developed internal organelles of a eukaryote.[ref]
Isolation of an archaeon at the prokaryote-eukaryote interface by Hiroyuki Imachi and others. Cultured MK-D1 morphology and proposed entangle–engulf–endogenize model
The evidence establishes plausibility of some components, not the order of every ancestral membrane event.The lipid divide adds a biochemical problem: typical archaeal membranes and typical bacterial/eukaryotic membranes differ in lipid linkage and glycerol stereochemistry. Replacement, coexistence or redistribution of lipid-synthesis pathways must be compatible with continuing membrane function; an abrupt wholesale replacement is not forced. Finally, membrane remodelling must be coupled to regulated protein targeting, metabolite exchange and division, so that the mitochondrion becomes an inherited endosymbiont and the new compartments persist. These requirements constrain any scenario even where the historical route remains uncertain.
Coat-associated adaptors couple three tasks: recognizing the correct membrane, selecting cargo, and assembling a carrier. Each interaction can be modest on its own; coincidence detection creates a selective assembly site. A sorting motif on a cargo's cytoplasmic tail can contact an adaptor directly, whereas soluble luminal cargo requires a transmembrane receptor to expose an adaptor-binding signal to the cytoplasm. Thus cargo recognition respects membrane orientation.
In clathrin-mediated endocytosis, the AP2 adaptor complex recognizes plasma-membrane determinants and cargo motifs while recruiting the clathrin scaffold. Other clathrin adaptors operate at internal membranes, so clathrin alone does not specify an itinerary. AP1 adaptor complex-associated carriers, for example, rely on a different local molecular context. Cargo, lipid and small-GTPase interactions collectively distinguish productive assembly from accidental coat binding.
COPII illustrates the same logic at endoplasmic reticulum exit sites. Membrane-associated Sar1 GTPase recruits the inner Sec23-Sec24 complex layer, in which Sec24 recognizes cargo and cargo receptors; Sec13-Sec31 complex builds an outer scaffold. COPI uses a different coat assembly, recruited by ARF-family GTPases, and participates in retrieval toward the endoplasmic reticulum and traffic within the Golgi apparatus. These systems need not have identical subunits to share the architecture of membrane recruitment, cargo selection and scaffold assembly.
An especially useful mechanistic test is biochemical reconstitution. Purified COPII coat components and defined liposomes were sufficient to produce coated vesicles, demonstrating that assembly itself can deform membranes rather than merely decorate carriers made by a wholly independent mechanism.[ref]
COPII-coated vesicle formation reconstituted with purified coat proteins and chemically defined liposomes by Ken Matsuoka and others. Reconstitution with Sar1, Sec23/Sec24 and Sec13/Sec31 on defined liposomes
Sufficiency in this minimal system does not imply that every regulator and cargo in a living cell is dispensable.Coat polymerization, membrane-inserting regions and accessory factors contribute to curvature, while fission machinery and details of neck geometry differ among pathways. The nucleotide cycles of Sar1 GTPase and ARF-family GTPases regulate coat recruitment and turnover; they should not be portrayed as identical engines executing every membrane-cutting step. After budding, substantial uncoating permits subsequent targeting and fusion. Destination specificity then depends on additional factors, including tethering machinery, Rab-family GTPases and SNAREs; a coat is not a complete postal address by itself.
To test the common design, mutate a cargo motif, its adaptor-binding site and the membrane-recruitment determinant separately. Measure recruitment, cargo concentration and productive transport as separate outputs, and rescue with the corresponding wild-type component. A cargo-selective defect without complete loss of carrier formation is particularly informative because it separates selection from the physical formation of a carrier.
Ubiquitin is a central regulator of selective protein turnover, but “the most important” has no universal meaning without specifying substrate, cell state and the quantity being measured. Selective destruction of a short-lived regulator, bulk recycling during starvation, and removal of a damaged mitochondrion are different problems. The ubiquitin system is extensive, yet it neither encompasses every degradation pathway nor makes all ubiquitination a destruction signal.
In the canonical pathway, an E1 enzyme uses ATP to activate ubiquitin, an E2 enzyme carries it, and an E3 ligase supplies much of the substrate specificity. Repeated conjugation can build chains on a substrate, while deubiquitinating enzymes edit or remove those modifications. Linkage and chain architecture influence recognition; a K48-linked chain is a common proteasomal signal, but “polyubiquitinated” does not specify a single outcome. Some ubiquitinations regulate location or signalling instead of degradation.
The proteasome recognizes suitable substrates, removes or recycles ubiquitin, unfolds accessible protein regions using ATP-dependent machinery, and threads the polypeptide into a proteolytic core. Substrate tagging is therefore one control point among several: accessibility, engagement and unfolding matter as well. This permits rapid removal of regulatory proteins and disposal of misfolded soluble proteins without digesting an entire organelle.
A particularly clear exception is ornithine decarboxylase. In a cell-free system, proteasome depletion blocked its ATP- and antizyme-dependent degradation; purified 26S proteasomes supported degradation without ubiquitin. This provides direct biochemical evidence that proteasomal destruction need not always require substrate ubiquitination.[ref]
Ornithine decarboxylase is degraded by the 26S proteasome without ubiquitination by Yasuko Murakami and others. Immunodepletion and purified-proteasome assays, Nature 360, pp. 597–599
It is a specific exception rather than evidence that ubiquitin is generally dispensable.Lysosomes provide another major route. Autophagy can sequester cytoplasm, aggregates and organelles in membrane carriers for lysosomal degradation. Some selective autophagy receptors recognize ubiquitinated cargo, so this route is partly coordinated with ubiquitin; bulk starvation-induced autophagy and other cargo-recruitment mechanisms show why it is not equivalent to proteasomal tagging. A yeast genetic screen used failure to accumulate autophagic bodies and failure of starvation-induced vacuolar protein turnover to identify autophagy-defective mutants. The experiment established a genetically separable membrane-delivery programme essential to this recycling response.[ref]
Isolation and characterization of autophagy-defective mutants of Saccharomyces cerevisiae by Miki Tsukada and Yoshinori Ohsumi. Mutant isolation, complementation groups, and nitrogen-starvation-induced vacuolar protein degradation
Membrane proteins can also be delivered through endocytosis and endosomal sorting, including ESCRT-dependent entry into internal vesicles before lysosomal destruction. Here ubiquitin often helps specify sorting, while receptor internalization, membrane traffic and lysosomal activity supply additional control points. Dedicated organellar proteases add further pathways.
Experimentally, compare proteasome inhibition, lysosomal inhibition and perturbation of a defined E3 ligase or autophagy factor while following a labelled substrate over time. A steady-state increase is insufficient: it can result from increased synthesis rather than reduced degradation. Measure turnover and pathway flux, check inhibitor toxicity and use genetic rescue. The defensible conclusion is that ubiquitin is a major, versatile selectivity signal whose importance is context-dependent; complete protein clearance depends on several regulated degradation systems.
Migration and admixture explain much of the broad genome-wide pattern, while drift, restricted mating and local demographic history generate finer structure; natural selection has disproportionately strong effects at particular loci. Mutation ultimately supplies new variation and genetic recombination creates new combinations, but neither alone explains the major spatial and historical contrasts among present-day European Homo sapiens populations. The relative importance depends on whether the target is genome-wide ancestry, a local population, or a specific adaptive trait.
The starting point is shared ancestry followed by differentiation, not a set of immutable European biological categories. Present populations are connected through repeated movements and reproduction, and much human variation occurs within any sampled population. Geographic clines can be real without implying sharp natural boundaries. Historical and linguistic labels identify sampling groups or hypotheses; they are not a substitute for analysing actual gene flow, allele frequencies and uncertainty in ancestry models.
Ancient DNA changed the historical explanation by making temporal replacement and mixture directly observable. Early genomic studies modelled present-day Europeans using contributions related to western hunter-gatherers, early farmers and ancient northern Eurasian ancestry. [ref]
Ancient human genomes suggest three ancestral populations for present-day Europeans by Iosif Lazaridis and others. Nature 513, pp. 409–413; ancestry mixture models and ancient reference genomes
These are statistical ancestry relationships to sampled ancient groups, not three pure, permanent ancestral races. Subsequent sampling has resolved additional structure and admixture within those sources. In particular, an early-farmer component must not simply be renamed a hunter-gatherer component because the farmer population already carried some admixed ancestry.The spread of farming brought substantial ancestry related to populations of Anatolia and neighbouring regions into Europe, followed by geographically variable mixing with resident hunter-gatherers. Later Neolithic and Bronze Age movements from the Pontic–Caspian steppe generated another major ancestry shift. Dated ancient genomes showed that some central European groups associated with the Corded Ware horizon had substantial steppe-related ancestry. [ref]
Massive migration from the steppe was a source for Indo-European languages in Europe by Wolfgang Haak and others. Nature 522, pp. 207–211; dated ancient genomes and late Neolithic ancestry change
These events provide a mechanism for coordinated changes at many unlinked loci. Similar pottery or a language family does not independently prove a one-to-one population replacement; the genetic, archaeological and linguistic claims require separate evidence.The elementary admixture calculation is:where are source allele frequencies and is the ancestry contribution under the stated two-source model. Many loci can move together without selection if their source frequencies differ. For an illustrative , and , . These invented values explain the logic rather than estimate any European ancestry. Further migration, drift and selection subsequently modify the mixture; imperfect ancient proxies also limit precision.
Genetic drift is particularly important after bottlenecks, colonization and prolonged small effective size. A founder effect samples only part of the ancestral variation, and subsequent growth can make initially unusual variants numerous without creating an adaptive advantage. Restricted movement, local mating networks and isolation by distance generate regional structure; continued gene flow generally counteracts divergence. An island, valley or relatively isolated community can therefore differ from neighbouring populations through demographic sampling rather than ecological adaptation. The relevant quantity is effective population size, which can differ greatly from the current census because of past size, reproductive inequality and mating structure.
Mutation supplies the alleles on which these processes act. Recent population growth also changes the abundance and age distribution of rare variants, so rare-variant contrasts need not reproduce the history inferred from common variants. Genetic recombination reshuffles ancestry and breaks down associations among loci. It does not directly change the frequency of an allele merely by exchanging chromosome segments, but its progressive shortening of ancestry blocks helps date mixture under an explicit demographic model. A single mitochondrial or Y-chromosomal genealogy gives a narrower history than the autosomal genome and can be especially sensitive to sex-biased movement or lineage loss.
Natural selection is essential for some conspicuous exceptions to a purely demographic account. Ancient-genome analyses identified changes involving pigmentation, diet and other traits, comparing observed frequencies with expectations given ancestry. [ref]
Genome-wide patterns of selection in 230 ancient Eurasians by Iain Mathieson and others. Nature 528, pp. 499–503; selection tests conditional on changing ancestry
A region unusually differentiated between populations is only a candidate: drift, a change of ancestry, correlated variants and the properties of the sampling procedure can all generate apparent outliers. Dated allele trajectories and comparison with an appropriate demographic null are much more informative than assuming that every geographic difference is an adaptation.Lactase persistence illustrates both strong selection and the need to distinguish competing causes. Dairying preceded the high frequency of adult milk digestion in many European populations. Archaeological dairy residues and ancient genetic time series indicate that milk use alone does not explain the allele's trajectory; hypotheses involving famine or infectious disease can change the advantage of lactose digestion. [ref]
Dairying, diseases and the evolution of lactase persistence in Europe by Richard P. Evershed and others. Nature 608, pp. 336–345; dairy residues, ancient allele frequencies and competing selective explanations
This is gene–culture coevolution, because cultural resource use changes the selective environment. It is not evidence that all people who consumed dairy were lactase-persistent or that every aspect of dairy adaptation arose from a new mutation after farming began.To compare the processes, I would fit demographic models to many relatively neutral regions, use ancient samples to test the timing and direction of ancestry changes, and then ask which loci deviate beyond plausible drift and sampling error. Contamination, damage, related individuals, uneven geographic coverage and imprecise dates need explicit treatment. A principal-component plot describes variation in a particular sample; it does not by itself identify an event or its cause. Likewise, an ancestry coefficient is conditional on the reference populations and model.
There is no single defensible percentage of European genetic differentiation attributable to each process. Migration and admixture are central to broad ancestry contrasts, drift and mating geography to local structure, and selection to particular functional differences. mutation creates the variation and recombination reorganizes it; these processes interact rather than replace one another.
Mammalian endothermy probably emerged through several interacting changes along the synapsid stem, and its precise onset remains disputed because the fossil proxies measure different aspects of physiology. Endothermy concerns substantial metabolic heat production; homeothermy concerns relatively constant body temperature. A large animal can have relatively stable temperature without a mammalian metabolic rate, while an endothermic animal can display heterothermy. These distinctions prevent a single temperature estimate or anatomical character from being treated as a complete diagnosis.
The physiological problem is a heat balance. In a deliberately simplified steady-state model:where is metabolic energy turnover, external work, effective thermal conductance of an animal, body and ambient temperature, and evaporative heat loss. Maintaining a warm body in a cool environment can involve increased metabolism, reduced conductance, behaviour, or a combination. For example, and a difference imply of non-evaporative heat loss in this illustrative model. The numbers are not a reconstruction of a fossil animal.
Along the synapsid lineage, increased sustained activity would require coordinated oxygen uptake, transport and use, greater food processing and sufficient energy assimilation. More effective locomotor construction, ventilation and circulation could support greater aerobic capacity, while insulation would reduce the cost of retaining the resulting heat. Shivering thermogenesis and later forms of non-shivering thermogenesis can contribute in living mammals. Brown adipose tissue in many living placental mammals cannot simply be assigned to early therapsids; a modern mechanism need not have been the ancestral one. Similarly, an expanded secondary palate or an altered limb posture is compatible with increased performance but is not a direct measurement of resting metabolism.
The time sequence must be reconstructed from several lines of evidence. Early synapsids lack the complete modern mammalian package, whereas various therapsids and cynodonts show changes in growth, feeding and respiratory anatomy before the mammalian crown radiation. Rapidly deposited fibrolamellar bone supports rapid growth, but fast-growing ectotherms and the influence of size and environment prevent a unique inference of endothermy. Growth interruptions can reflect seasonality or resource shortage rather than a categorical physiological boundary. Nasal structures interpreted as respiratory nasal turbinates could reduce water and heat loss during high ventilation, but identifying their precise form and separating respiratory from olfactory roles in fossils is difficult.
Preserved hair supplies direct evidence of insulation in some later fossils. Castorocauda, a Middle Jurassic mammaliaform, preserves integument alongside an aquatic anatomical specialization. [ref]
A swimming mammaliaform from the Middle Jurassic and ecomorphological diversification of early mammals by Qiang Ji and others. Science 311, pp. 1123–1127; Castorocauda skeleton and preserved integument
This establishes that a fur-bearing covering existed by that time, not when insulation first evolved or whether its original function was thermal. Sensory and protective functions can precede elaboration for heat conservation. Direct preservation is particularly valuable, but its late appearance in the sampled record is not proof of biological absence in older lineages.Stable isotope analysis has suggested earlier elevated thermometabolism. Comparing oxygen-isotope compositions of therapsid apatite with those of coexisting tetrapods, one study inferred differences in physiology and proposed elevated thermometabolism in several Permo-Triassic therapsid groups. [ref]
Oxygen isotopes suggest elevated thermometabolism within multiple Permo-Triassic therapsid clades by Kévin Rey and others. eLife 6, e28589; therapsid apatite compared with coexisting tetrapods
The comparison is stronger than analysing one isolated animal because coexisting taxa constrain aspects of the environment. Nevertheless, body water, drinking source, habitat, evaporation and diagenesis affect the isotopic signal. The proposed middle-to-late Permian origin is an interpretation using a physiological framework, not a thermometer reading of an observed living cynodont.A contrasting biomechanical approach uses the temperature dependence of endolymph properties and the dimensions of the semicircular canals. Calibration against living animals and application to fossil inner ears supported a relatively abrupt transition around 233 million years ago in the Late Triassic, near the origin of mammaliamorphs. [ref]
Inner ear biomechanics reveals a Late Triassic origin for mammalian endothermy by Ricardo Araújo and others. Nature 607, pp. 726–731; living-species calibration and inferred transition around 233 Ma
This offers a quantitative prediction from a different anatomical system. However, body size, activity, reconstruction and the adequacy of the living calibration remain relevant. A change in a temperature-sensitive inner-ear proxy need not coincide exactly with the first increment in metabolic heat production or the first insulating covering. The disagreement with earlier isotope-based interpretations should therefore be tested, rather than erased by choosing the preferred date.There are several plausible selective explanations. The aerobic capacity hypothesis proposes that selection for sustained locomotor performance raised maximum oxygen consumption, with elevated resting metabolism and heat production linked to that change. Comparative measurements of resting and maximum oxygen use underpin this proposal. [ref]
Endothermy and activity in vertebrates by Albert F. Bennett and others. Science 206, pp. 649–654; resting and maximum oxygen consumption and the aerobic-capacity hypothesis
A major issue is the strength and evolutionary direction of the relationship: high resting expenditure is expensive, and an association among living species does not prove which change led historically. Selection for thermal independence, nocturnal activity or performance in fluctuating climates provides related benefits, but “the climate became colder” is not sufficient unless the energetic costs and available food are considered.A parental care hypothesis instead emphasizes selection for controlling the developmental environment and supplying offspring. Improved provisioning endurance and more stable incubation or offspring temperatures could favour increased metabolic capacity and heat retention. [ref]
Parental Care: The Key to Understanding Endothermy and Other Convergent Features in Birds and Mammals by C. G. Farmer. The American Naturalist 155, pp. 326–334; parental-care hypothesis
This gives concrete reproductive benefits that might offset energetic costs, while remaining a hypothesis about historical selective circumstances. The evidence required includes relationships among care, thermal performance and reproductive success, not merely the fact that living mammals both care for young and are endothermic. Activity, parental investment, insulation and environmental variability could reinforce one another, so the explanations need not be mutually exclusive.The most secure account is a mosaic physiological transition with increasingly effective energy supply, heat production and heat retention. A Late Triassic onset of a more fully mammalian condition is a specific supported hypothesis, while earlier therapsid evidence indicates that parts of the transition may be older. fossil anatomy and chemistry constrain when particular features existed; the selective reasons require functional and comparative tests and remain less directly observable.
Skeletal anatomy can reconstruct likely resource use and test hypotheses about competition, but it cannot by itself measure the strength of an interaction between fossil populations. Resource partitioning among living sympatric primate species provides a useful source of comparative predictions. It does not establish that every difference among coexisting fossil species was caused by competition: differences may predate coexistence, reflect other selective pressures, or merely determine which species can occur together.
The first requirement is to establish the relevant community. fossils from one formation may have accumulated over many thousands of years or represent animals transported from different habitats. Stratigraphy, dating, sedimentology and taphonomy must therefore establish plausible coexistence at an ecologically relevant scale. Species boundaries, skeletal associations, age, sex and the number of individuals also need attention. A mixed collection of several time-separated populations cannot be treated as one living primate group, and an isolated limb should not be confidently assigned to a hominin species solely because its teeth occur nearby.
For diet, I would measure tooth size and proportions, crown shape, shearing edges, enamel thickness, jaw geometry and muscle attachment regions. Functional morphology connects these observations to potential food processing: slicing leaves, crushing relatively hard items and resisting repeated chewing loads impose different demands. Body size affects both mechanics and energetic requirements, so comparisons need allometry rather than assuming that a larger tooth necessarily reflects a different food category. Phylogenetic relationships also matter because inherited resemblance can produce apparent ecological overlap independently of recent competitive interactions.
These measurements estimate capability better than habitual consumption. Paranthropus boisei has a powerful chewing apparatus and very large postcanine teeth, yet a dental-microwear study found comparatively low surface complexity and anisotropy in the seven specimens preserving suitable surfaces. [ref]
Dental Microwear and Diet of the Plio-Pleistocene Hominin Paranthropus boisei by Peter S. Ungar and others. PLoS ONE 3, e2044; seven specimens with preserved microwear and comparison with gross anatomy
This contradicted a straightforward inference of habitual hard-object feeding from robust anatomy alone. It is compatible with the importance of mechanically demanding fallback foods, or other uses of the apparatus, without uniquely demonstrating either explanation. A morphology selected during rare food shortages need not correspond to the last meals recorded by dental microwear.Enamel chemistry provides a partially independent test. Carbon-isotope measurements indicated substantial use of C4-based resources by Paranthropus boisei. [ref]
Diet of Paranthropus boisei in the early Pleistocene of East Africa by Thure E. Cerling and others. PNAS 108, pp. 9337–9341; enamel carbon isotope evidence for C4-based resources
This helps distinguish it from a consumer relying predominantly on C3-derived resources, but does not specify the plant part, exact food species or necessarily every intermediate step through a food web. Grasses and sedges can share the broad photosynthetic signature. Isotopic overlap therefore need not mean identical diets, just as different wear patterns need not imply complete separation. The strength of the reconstruction comes from combining evidence that integrates different biological timescales and different aspects of resource use.For locomotion, I would examine joint shape, limb proportions, phalangeal curvature, grip-related structures, the shoulder, pelvis, vertebral column and articular surfaces. These can constrain leaping, climbing, suspension, quadrupedal walking or habitual bipedalism and hence access to canopy levels, support diameters and terrestrial resources. However, a locomotor category is not a diet. Animals with similar locomotor competence may choose different foods, while animals with different locomotion may compete for the same ground-level resource. Wear, preservation and reconstruction uncertainty need to be propagated rather than assigning every specimen to a single categorical lifestyle.
Hominins make this caution especially important. A bipedal lower limb need not imply complete abandonment of climbing. Comparative analysis of the juvenile scapula of Australopithecus afarensis supported retained climbing-related features and showed why ontogeny matters in comparison with living apes. [ref]
Australopithecus afarensis scapular ontogeny, function, and the role of climbing in human evolution by David J. Green and others. Science 338, pp. 514–517; juvenile scapula and comparative growth patterns
This informs possible resource access, but does not quantify time spent climbing or competitive effects on another species. A fossil community containing an australopith, a species of Homo and other primates could consequently share some resources while partitioning others. The anatomical mosaic should be retained in the model rather than compressed into a single “terrestrial” score.An explicit model clarifies what is missing. In one conventional competition model: is an ecological competition coefficient, defined relative to the chosen density units and model assumptions. It represents the effect of another population on population , not simply their morphological resemblance. Estimating it requires information about density, resource limitation and demographic responses that skeletal shape rarely provides. The same niche overlap could accompany negligible competition when food is abundant and severe competition during a bottleneck. Conversely, strong present-day partitioning could be a legacy of past competition rather than evidence that competition was always weak.
I would therefore construct quantitative, uncertainty-aware estimates of dietary and locomotor overlap, calibrated against living primates with measured behaviour. The calibration should include species occupying similar environments but differing in abundance or competitive context, and test predictions on species excluded from model fitting. A morphospace can summarize measurements, but distance in it is not automatically ecological distance. Closely related species, correlated skeletal measurements and multiple teeth from one individual cannot be counted as independent demonstrations.
To test competition more directly, compare putatively interacting species across intervals or localities with and without the competitor, while accounting for habitat, climate, ancestry and body size. Divergence specifically associated with overlap would support ecological character displacement more strongly than a difference observed at one site. Comparable shifts in abundance, resource availability or population performance would strengthen the inference, although fossil abundance itself is affected by preservation and collection. Several independent lines of evidence are needed to distinguish competition from environmental filtering or an inherited ecological difference.
The outcome should be a ranked set of hypotheses about which resources were potentially shared, when limitation was plausible and whether divergence is associated with coexistence. Skeletal differences can support partitioning and make competition explanations testable; neither similarity nor difference alone is a direct measure of competitive strength.
Introduced mammals have affected native populations through predation, competition, disease, habitat modification and hybridization; mitigation works best when it targets the demonstrated mechanism at the geographic scale of reinvasion. Britain and Ireland must be assessed separately, and native status is local. A mammal native to mainland Britain can be an introduced species on an offshore island. An introduced population is not automatically an invasive species: establishment, spread and adverse effects need evidence.
Grey squirrels, introduced in Victorian Britain and subsequently Ireland, illustrate several mechanisms. Their expansion has accompanied major contraction of red squirrels, involving resource competition as well as pathogen-mediated effects in some regions. Experimental infection found severe disease in red squirrels and little detectable effect on grey-squirrel health, supporting a role for squirrelpox. [ref]
Parapoxvirus causes a deleterious disease in red squirrels associated with UK population declines by Daniel M. Tompkins and others. Proceedings of the Royal Society B 269, pp. 529–533; contrasting experimental susceptibility of red and grey squirrels
That comparison establishes differential susceptibility, not the cause of every field decline. Habitat, exposure, squirrel density and the presence of the virus must be assessed locally. grey squirrels also damage trees through bark stripping, adding forestry costs to biodiversity effects.A response can combine surveillance, exclusion of new introductions, targeted population control and habitat management favouring red squirrels. Control should be coordinated across connected populations because small cleared areas can be repeatedly recolonized. Recovery of pine martens in Ireland has been associated with reduced grey-squirrel abundance, making predator recovery a potentially useful part of management. [ref]
Population crash in an invasive species following the recovery of a native predator: the case of the American grey squirrel and the European pine marten in Ireland by Emma Sheehy and others. Biodiversity and Conservation 23, pp. 753–774; distributional changes associated with pine marten recovery
The association is not a guarantee that every woodland will respond similarly or a reason to ignore effects on other prey. Predator recovery and direct squirrel management should be evaluated through measured outcomes and the local ecological setting.American mink, established through twentieth-century escapes and releases associated with fur farming, have affected vulnerable prey, including water voles and some waterbirds. Their movements along waterways make isolated trapping effort vulnerable to reinvasion from elsewhere. Landscape-scale coordinated monitoring and removal in Scotland showed how volunteer participation and adaptive deployment can operate at a much larger scale than occasional local control. [ref]
Turning back the tide of American mink invasion at an unprecedented scale through community participation and adaptive management by Rosalind Bryce and others. Biological Conservation 144, pp. 575–583; landscape-scale monitoring and coordinated control
A trap capture is an operational measure; the conservation endpoint is improved prey survival, occupancy or reproduction. Habitat restoration remains important where bank condition, fragmentation or other pressures also limit water voles.Introduced deer create a different set of impacts. Sika deer and muntjac can contribute to heavy browsing, changes in woodland regeneration and understorey structure, damage to crops and increased collision risk. Attribution needs care because native deer and changes in their abundance can contribute to the same pressures. In an English woodland experiment, paired fenced and browsed areas of coppice provided evidence that deer exclusion altered habitat use by breeding nightingales. [ref]
Experimental evidence that deer browsing reduces habitat suitability for breeding Common Nightingales Luscinia megarhynchos by Chas A. Holt and others. Ibis 152, pp. 335–346; eight paired deer exclosures and browsed controls
Pairing helped separate browsing effects from much of the shared habitat setting, but the experiment did not assign all landscape-level bird decline to introduced deer alone. Deer management should therefore use observed vegetation and wildlife responses rather than a target justified solely by species origin.Sika deer also hybridize with native red deer. Genetic analysis of a Scottish contact zone detected introgression even though many animals remained readily classified as red-like or sika-like. [ref]
Introgression through rare hybridization: A genetic study of a hybrid zone between red and sika deer (genus Cervus) in Argyll, Scotland by Simon J. Goodman and others. Genetics 152, pp. 355–371; microsatellite and mitochondrial evidence of introgression
Phenotypic appearance therefore cannot reliably exclude mixed ancestry. The genetic objective of management must be stated explicitly, with appropriate sampling and markers; local removal cannot undo past gene flow already distributed through a population. Preventing further releases or escapes and managing contact zones can be more tractable than claiming that every admixed individual can be identified visually.Offshore islands show why national native status is insufficient. Introduced hedgehogs in the Western Isles became predators of wader eggs. A removal experiment compared fenced plots with adjacent controls and found improved nest success where hedgehogs were removed, without evidence that native bird predators compensated fully for the reduction. [ref]
Experimental removal of introduced hedgehogs improves wader nest success in the Western Isles, Scotland by Digger B. Jackson. Journal of Applied Ecology 38, pp. 802–812; fenced removal plots, adjacent controls and nest monitoring
This supplies stronger causal evidence than a simple correlation between hedgehogs and declining birds. Exclosures and removal can protect critical sites, but fence maintenance, recolonization and the consequences of moving animals elsewhere must be considered. Transporting a problem to another sensitive site is not effective mitigation.Ireland also has recent small-mammal invasions. The greater white-toothed shrew, first recorded there in 2007, expanded in a region previously occupied by the native pygmy shrew; field studies linked the invasion to changes in the latter's distribution. [ref]
Invading and expanding: range dynamics and ecological consequences of the greater white-toothed shrew (Crocidura russula) invasion in Ireland by Allan D. McDevitt and others. PLoS ONE 9, e100403; first recorded in 2007, spread and native pygmy-shrew distribution
The finding motivates monitoring invasion fronts and native populations, while recognizing that distributional association alone does not completely identify the competitive mechanism. Small species are easily moved unnoticed with materials, so pathway surveillance can be valuable even where widespread eradication is difficult. A British management priority cannot simply be copied to Ireland because the native communities and invasion histories differ.Eradication is possible under suitable conditions. The British campaigns against muskrats and coypus, both introduced through fur farming in the 1920s, illustrate the importance of early response and sustained demographic planning. Later coypu control used population studies, trapping-effort information and coordinated deployment rather than assuming that opportunistic captures would finish the job. [ref]
The eradication of muskrats and coypus from Britain by L. M. Gosling and others. Biological Journal of the Linnean Society 38, pp. 39–51; contrasting campaigns and population-based control planning
The lesson is operational as well as ecological: eradication requires resources to find the last animals, a reason for participants to continue as captures decline, and surveillance after apparent success.Across examples, prevention and rapid response are usually more feasible than reversing a widespread established invasion. Measures include securing managed animals, identifying transport pathways, detecting new populations promptly and selecting geographically defensible management units. Where complete eradication is unrealistic, sustained suppression or protection of high-value sites may still have substantial benefits. Methods should minimize harm to non-target animals and be compared for effectiveness, feasibility and welfare consequences. Reinvasion, compensatory reproduction and interactions among predators or competitors can otherwise undermine a superficially successful intervention.
Evaluation should use appropriate controls or a before-after control-impact design, with detection effort and habitat change recorded. Reduced invader abundance, improved native reproduction, recovered vegetation and reduced introgression are distinct outcomes and may not change together. Successful mitigation is not simply fewer introduced animals: it is a demonstrated reduction of their harmful effects, maintained through appropriate geographic coverage, prevention of renewed introductions and continued monitoring.
Articles were limited to the first 100 out of 168 total.
Articles by others on the same topic
There are currently no matching articles.