Orientation selectivity is a systematic dependence of a visual neuron's response on the axis of a bar, edge or stripe pattern presented in its receptive field, under specified stimulus conditions. Here the angle measures the stripe axis from horizontal: is horizontal and vertical. An axis has no arrow, so and describe the same orientation. A preference for one direction of movement across that axis is an additional property; the 1962 recordings included both equal and unequal responses to opposite movements. [ref]
https://www.gatsby.ucl.ac.uk/teaching/courses/tn1-2020/additional/systems/JPhysiol-1962-Hubel-106-54.pdf. Hubel and Wiesel (1962), p. 112: orientation versus opposite movements
A particularly clear experiment using extracellular single-unit recording appears in the 1959 paper, Figures 2–3. A bright slit was centered on the same receptive field and rotated through successive angles; each presentation lasted one second. The vertical slit strongly increased the extracellularly recorded spike train, whereas the horizontal slit was ineffective. Small-spot tests had identified ON and OFF receptive-field subregions, with a central ON region and opposing flanks: rotation illuminated less of the center and more of the flanks. Geometry and location therefore mattered together. These dimensions belong to that recorded unit, not to every neuron. [ref]
https://xbio-live.s3.amazonaws.com/narratives/57358/Hubel%20and%20Wiesel%201959_Guided%20paper.pdf. Hubel and Wiesel, Receptive fields of single neurones in the cat's striate cortex (1959), pp. 578–579, Figures 2–3: primary recordings
An orientation tuning curve summarizes a controlled angle sweep. Keep location, size and visual contrast fixed; for a stripe pattern also specify spatial frequency and phase. The same signed spatial filter model of a simple cell can produce strong orientation selectivity and strong dependence on phase, as the following original toy illustrates. Its smooth curves are calculated predictions, not digitized or invented biological measurements.
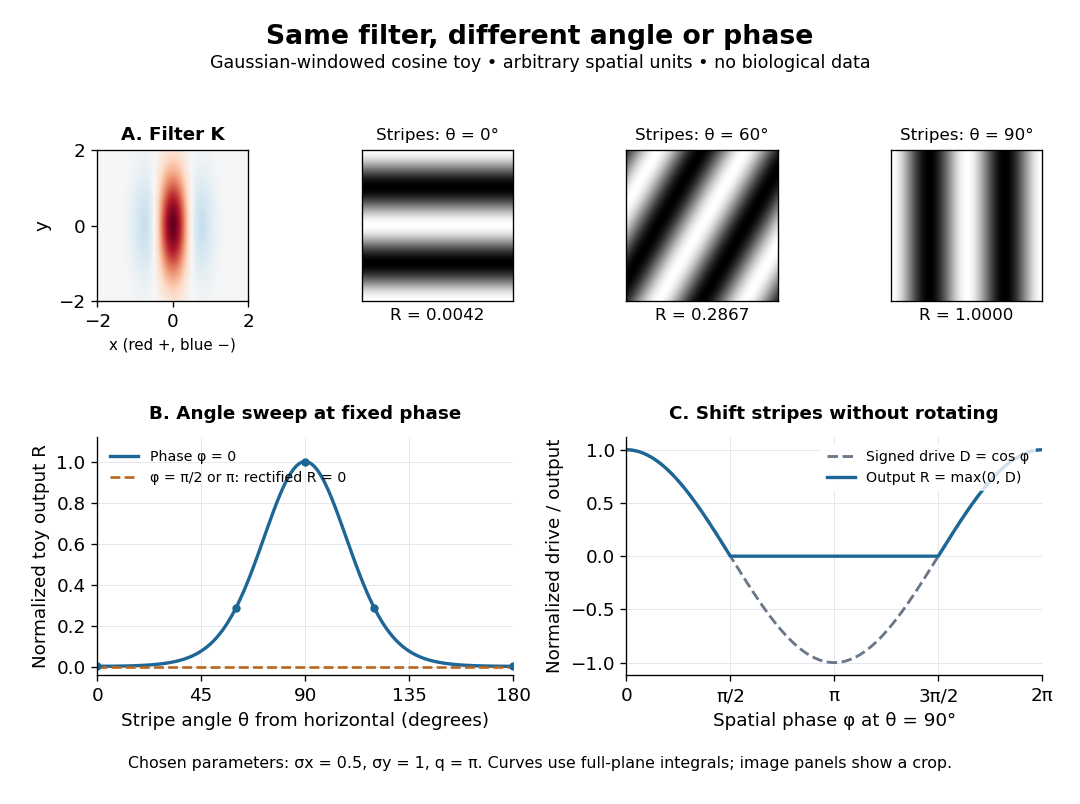

An orientation tuning curve plots a specified response against the stimulus-axis angle , with the other stimulus variables controlled. A practical count summary for extracellular single-unit recording iswhere counts action potentials in the same duration on trial , and is the number of repeats at each angle. This estimates spikes per unit time in that window; the window must specify whether it covers onset, sustained stimulation, or both. Record a blank-background response separately, and report whether it has been subtracted. Randomizing angle order and repeating each condition helps separate orientation selectivity from changes over time, including neural adaptation. This is a proposed measurement procedure, not a claim that the original experiments used this estimator.
A simple cell's orientation tuning curve can also change when the stimulus shifts. An angle sweep at fixed phase, a sweep averaging over phase, and a sweep of moving stripes ask different questions. Consequently, a single preferred angle does not specify the whole receptive field. The toy curve under orientation selectivity holds phase fixed and plots dimensionless output, rather than spikes per second.
Correlation-based learning among spatially arranged ON and OFF inputs, with synaptic competition and lateral interactions, can select elongated simple cell receptive fields. Neighbor interactions coordinate preferred orientations across cortex, while competition allows different orientations to persist. Selectivity within one cell and a spatial map across many cells are separate predictions, and neither follows from unbounded Hebbian learning alone.
Articles by others on the same topic
There are currently no matching articles.