Let be prey and predator abundances. With constant positive demographic and predation coefficients, the Lotka-Volterra equations areTheir positive equilibrium is , . Its Jacobian matrix and eigenvalues areThe linearized populations oscillate with period , with the predator peak following the prey peak. This is a center equilibrium, not an attracting equilibrium. The conclusion is supported beyond linearization by the Logarithmic first integral of the Lotka-Volterra equations: in these units one may useDirect differentiation gives . Its Hessian matrix is a positive-definite matrix in the positive quadrant, and its minimum is at . Nearby level curves are closed periodic orbits, so there is no damping toward a preferred oscillation amplitude.
Use an annual pulse-breeding predator-prey model. Let be the abundances just after reproduction, and let the year have length . Between breeding pulses, assume mass-action predation, natural mortality rates , and no reproduction:Solving the predator equation and inserting it into the prey equation gives the pre-breeding abundancesSuppose reproduction multiplies surviving prey by and adds offspring per surviving predator. Retaining the surviving adults gives , . Define , , and . The resulting difference equations areThus offspring depend on prey available at the end of the year, not on the number killed during the year. The adult-survival convention is part of the model; if breeding replaces all adults, use instead. Both are consistent pulse models under their respective life-history assumptions.
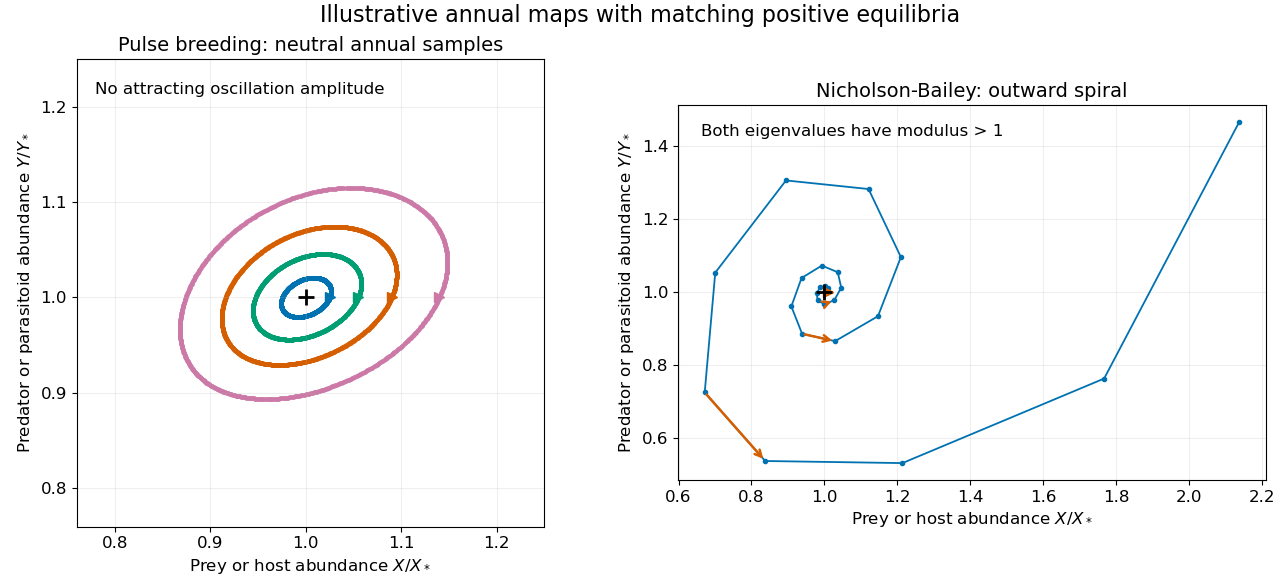
For the adult-survival annual pulse-breeding predator-prey model, a positive annual fixed point exists when and :At this point the Jacobian matrix isIf , the two eigenvalues are a complex conjugate pair of moduli one. The annual samples show linearly neutral seasonal oscillations. If , they form a reciprocal negative real pair and the fixed point is a saddle fixed point of a map. Equality at four is a degenerate boundary needing nonlinear analysis. For replacement rather than surviving adults the same calculation gives trace and determinant one.
The absence of an attracting annual cycle is stronger than a linear observation. Put , . The update becomesIt is the composition of two nonlinear shear maps, each of determinant one: an area-preserving seasonal predator-prey map. No isolated positive periodic orbit has an open attracting basin. Neutral linear oscillations alone also do not prove nonlinear stability at every resonance. In particular, this density-independent model does not select an asymptotically stable oscillation amplitude.
The Nicholson-Bailey model instead counts parasitoid offspring from attacked hosts:Its positive equilibrium has and . Its Jacobian matrix hasSince the determinant exceeds one while the positive trace is below two, the eigenvalues are complex with moduli greater than one: instability of the Nicholson-Bailey equilibrium produces outward oscillations near it. The two maps share an exponential prey-survival factor but have different reproduction laws and stability properties.

Articles by others on the same topic
There are currently no matching articles.