Study answers to every option in the clinical social cognition examination of 25 May 2022. Source release: released examination PDF. The original examination required a choice of three; this resource covers all six without reproducing the statements.
Scientific claims use evidence available by the examination date. Diagnostic groups, individual cognitive profiles and causal mechanisms are distinguished; illustrative calculations are not experimental measurements.
Theory of mind and affective empathy are partly dissociable psychological capacities, while cognitive empathy overlaps substantially with mental-state understanding. A person can understand that another has a mistaken belief without sharing the person’s emotion; conversely, another’s distress can elicit an affective response without accurate reasoning about its cause. These possibilities do not establish wholly independent modules. The central question is which operations, measurements and circumstances can be separated.
Theory of mind concerns representing mental states such as beliefs, knowledge, desires and intentions. It can include non-emotional content: predicting where someone will search after an unseen object transfer need not involve feeling that person’s disappointment. Affective empathy involves sharing aspects of another’s affect with a self-other distinction. Cognitive empathy concerns understanding another’s emotional perspective and therefore recruits some of the operations also called theory of mind. Compassion, the concern that motivates helping, is different again; personal distress can be intensely aversive to the observer without yielding accurate understanding or useful assistance. Whether “empathy” dissociates from mentalizing consequently depends partly on which component is meant.
Psychological dissociation requires more than two differently named tasks. A belief story also demands language, working memory and response selection; a pain picture demands visual attention and interpretation. Differences between a story test and an emotional-rating scale could therefore reflect task impurity. A single correlation is equally inconclusive: shared verbal skill or a general tendency to endorse questionnaire items can create apparent unity. Conversely, noisy measurements can conceal a genuine association. The strongest designs measure both constructs within the same people, distinguish their target demands and include independent measures of validity.
The EmpaToM paradigm provides a useful example. Short autobiographical videos varied emotional content independently of whether a subsequent question required mental-state inference or factual reasoning. Affect and compassion ratings were obtained separately from reasoning performance. In the large validation experiment, the corresponding behavioural indices related selectively to activity in distinguishable networks, including anterior insula for affect sharing and temporoparietal regions for mentalizing. This supports separability within one task framework, rather than relying solely on unrelated literatures. It does not establish that the constructs never interact or that their measurement is perfectly pure.[ref]
Dissecting the social brain: Introducing the EmpaToM to reveal distinct neural networks and brain-behavior relations for empathy and Theory of Mind by Philipp Kanske and others. Abstract and Experiments 1–2, pp. 6–19: factorial manipulation, behavioural validation and selective brain–behaviour relationships
Earlier imaging studies help specify the contrast. A self/partner pain experiment identified shared affect-related activity without identical recruitment of every sensory component of directly experienced pain. Belief-story experiments contrasted mental representation with nonmental representation, rather than merely contrasting people with objects. Together these findings suggest different component computations; overlapping or distinct blood-oxygenation signals cannot alone establish psychological identity or independence. An anatomical label is not a definition of empathy, and activating a region implicated in several processes cannot uniquely diagnose which process occurred.[ref]
Empathy for pain involves the affective but not sensory components of pain by Tania Singer and others. Abstract: self-pain versus partner-pain conditions and affective/sensory contrasts
[ref]People thinking about thinking people: the role of the temporo-parietal junction in theory of mind by Rebecca Saxe and others. Experiments 1–2: belief versus nonmental-representation controls
Lesion evidence can strengthen the inference. A study comparing inferior-frontal and ventromedial-prefrontal lesions reported different patterns of emotional and cognitive empathy impairment, a behavioural double dissociation. That pattern argues against a simple single ability differing only in overall difficulty. However, lesions affect networks as well as local tissue, groups can differ in lesion extent, and the measures operationalize particular components rather than all possible mental-state understanding. The result supports multiple contributions, not a claim that one region contains every affective response and another every social inference.[ref]
Two systems for empathy: a double dissociation between emotional and cognitive empathy in inferior frontal gyrus versus ventromedial prefrontal lesions by Simone G. Shamay-Tsoory and others. Abstract and pp. 617–627: lesion-group comparison and cognitive/emotional empathy measures
Atypical development also makes confounding visible. In an empathy-for-pain study, insula responses tracked alexithymia across autistic and non-autistic participants rather than diagnostic group after adjustment. This challenges the inference that a difficulty in one aspect of social cognition necessarily entails an absence of affect sharing. It remains correlational evidence, and a nonsignificant adjusted group difference is not a proof of exact equivalence.[ref]
The capacities can nevertheless cooperate. Understanding that someone is grieving can direct attention toward relevant cues; sharing discomfort can motivate further inquiry into its cause. An observer’s own emotion may also bias interpretation, so stronger affect is not guaranteed to produce more accurate mentalizing. Accurate understanding can support compassionate help or strategic manipulation depending on motivation. These examples distinguish computational interaction from identity: two processes can causally influence one another without being the same process.
The distinction between capacity and spontaneous deployment is especially important. An explicit instruction may elicit reasoning that would not occur automatically in a distracting interaction. A person can also understand another’s state while declining to report an emotion, or feel concern while finding a questionnaire difficult. Better tests combine accuracy, ratings, behavioural choices and physiological measures, while checking reliability, language demands and response bias. Training or perturbation should produce a selective change on independently validated outcomes before being taken as evidence of a psychological separation.
The justified conclusion is therefore graded. Mental-state representation, affect sharing, compassionate concern and self-directed distress can be distinguished conceptually and empirically, with converging task, imaging and lesion evidence. The strongest dissociation concerns mentalizing and affect sharing, rather than every use of the word empathy. Real interactions recruit these components together with attention, learning and motivation; explaining that coordination is more informative than either treating all social understanding as one ability or assuming completely insulated systems.
Mirror neurons provide an observation–execution matching property that can contribute to action processing; their existence does not establish one exclusive function such as reading intentions. Plausible roles include linking seen actions to motor representations, predicting familiar action sequences and supporting imitation. The evidence is strongest when a specified task, representation and causal contribution are identified, and weaker when every social capacity is attributed to a broadly defined mirror system.
The original evidence was unusually direct. Single-neuron recordings in macaque premotor area F5 identified cells active both when the animal performed an action and when it observed a related action. Some observation–execution relations were relatively specific, whereas others generalized across aspects of the act. This is evidence about individual recorded cells, rather than merely overlapping brain regions. Yet the experimenter’s action label does not tell us exactly what the cell encodes: movement, object interaction, learned outcome and context can covary.[ref]
Action recognition in the premotor cortex by Vittorio Gallese and others. Summary and pp. 593–609: macaque F5 recordings and observation–execution congruence
An important extension tested incomplete visual information. Some cells responded when the final object interaction was hidden but could be inferred from the preceding situation. Thus a full visual display of the critical movement was not always necessary for activation. This is compatible with an internally generated action representation or prediction. It is not proof that a neuron understands another person’s beliefs, nor that the representation is generated without input from other visual or contextual systems. Familiar-context prediction and mental-state attribution are distinguishable hypotheses.[ref]
I know what you are doing: a neurophysiological study by Maria Alessandra Umiltà and others. Abstract and pp. 155–165: responses during visible and occluded action completion
Human evidence requires care about measurement scale. Functional imaging showing activation during both action observation and execution can involve different cell populations within one voxel. A motor-evoked potential during observation measures a downstream excitability change, not one cell’s selectivity. Intracranial recordings in a clinical epilepsy sample did identify individual observation–execution matching responses, including in supplementary motor and medial-temporal regions. That establishes relevant human cellular responses in the sampled tissue. Electrode placement was clinically determined, however, so it does not supply a representative census of the putative inferior-frontal/parietal system or of the general population.[ref]
Single-neuron responses in humans during execution and observation of actions by Roy Mukamel and others. Abstract and Experimental Procedures: individual-unit responses, clinical sample and electrode-placement constraints
A functional claim then needs a task contrast. Recognizing that a hand grasps an object, anticipating how a lift will unfold, judging the object’s weight and understanding a deceptive intention are not interchangeable forms of “action understanding.” Matching circuitry could improve one without being necessary for all. It may supply motor predictions that combine with visual object knowledge and contextual inference. Calling every successful judgment simulation would make the hypothesis difficult to falsify; the account must predict a deficit or response pattern that alternatives do not predict.
A stimulation experiment addressed a narrower causal question. Disrupting left inferior frontal cortex impaired judgments of a box’s weight from a person lifting it, with comparison tasks involving a bouncing ball and stimulus duration and comparison stimulation sites. These controls strengthen the inference that this region contributes to interpreting the action under those conditions. The manipulation still affected a cortical region, not selectively its mirror neurons. It therefore cannot establish that mirror cells are the sole mechanism, or that the region is necessary for all conceptual understanding of actions.[ref]
Action understanding requires the left inferior frontal cortex by Gorana Pobric and others. Summary and Results, pp. 524–529: weight judgments, nonhuman-motion/duration controls and stimulation sites
Developmental origin is a separate question from present function. In counter-mirror training, participants repeatedly performed one finger action while observing another. Subsequent muscle-specific responses to motor-cortex stimulation changed from the usual matching pattern toward the trained mismatching relation. This supports experience-dependent calibration of the action-observation/motor relationship. It challenges an account in which every relevant mapping is fixed and independent of experience, while leaving open contributions from developmental constraints. The measure was a motor-evoked response, so the experiment did not directly reprogramme an individually recorded mirror cell.[ref]
Sensorimotor learning configures the human mirror system by Caroline Catmur and others. Abstract and pp. 1527–1531: pre/post training muscle-specific responses and reversed sensorimotor pairing
This evidence also separates function from adaptation. A learned matching circuit may currently assist prediction or action selection even if it was not selected by evolution specifically to understand minds. Conversely, showing a plausible contribution to imitation does not show that every matching response exists for imitation. The same representation can be used in several tasks. Evolutionary stories require comparative or developmental evidence beyond the presence of useful response properties in an adult laboratory preparation.
Broad clinical explanations supply further tests. In one child study, several goal-imitation and action-representation measures were preserved in autistic participants despite poorer theory-of-mind performance. These behavioural results argue against a universal loss of action matching explaining every social difficulty. They do not demonstrate normality of every mirror population, because cells were not directly recorded. The important inference is that different social tasks cannot be assumed to stand in for one another.[ref]
The most defensible functional account is therefore contributory and conditional. Matching responses provide a route by which action observation can access action-related representations; learning, context and task goals determine how those representations are used. Single-cell recordings establish the property, controlled training tests plasticity, and well-designed perturbations test task-specific necessity. A comprehensive theory must connect all three while allowing other systems to supply object knowledge, language, attention and mental-state inference. Existence, selectivity, developmental origin and behavioural usefulness are four questions, not four names for the same finding.
Imitation requires a usable mapping from another person’s perceived action to one’s own action system, together with retention, selection and execution appropriate to the task. It does not invariably require explicit theory of mind, verbal instruction or conscious intention to copy. Those processes can organize sophisticated imitation, but simple action matching can occur without them. The first requirement is therefore to establish what was copied and exclude alternative routes to a similar response.
An observer may reproduce an action’s bodily form, its sequence, its object-directed goal or only its environmental outcome. Producing the same outcome by another means is emulation rather than clear evidence of copying the demonstrated movement. Increased object exploration after watching another person is weaker still. A convincing task therefore needs baseline performance and demonstrations that distinguish candidate targets: two demonstrators achieving one goal differently, or the same movement producing different outcomes. Without such contrasts, successful performance does not identify the representation that guided it.
The motor correspondence problem is fundamental. The observer sees another body from an external perspective but controls their own body through motor commands and proprioceptive feedback. Copying a finger lift or facial gesture requires some relation between these different descriptions; literal duplication of retinal coordinates is not enough. A mirror-like spatial response and an anatomical response can even require opposite transformations when facing another person. A system that copies goals can use existing action elements to assemble a new sequence without already possessing a complete motor programme for that sequence.
Experience offers a mechanism for acquiring these relations. Seeing one’s own movements, acting together with others and observing other people imitate oneself can correlate visual and motor events. Counter-mirror training demonstrated that deliberately mismatching observed and executed finger actions changes subsequent matching-related motor responses. Thus correspondence is at least partly learnable. This finding does not prove that all imitation is acquired by the same process or that newborn action matching is impossible; it identifies a concrete source of plasticity in adults.[ref]
Sensorimotor learning configures the human mirror system by Caroline Catmur and others. Abstract: sensorimotor training changes the observation–execution relationship
Automatic imitation experiments isolate one consequence of a mapping. Participants make an instructed finger movement while an irrelevant observed movement is compatible or incompatible with it. Observed action identity influences performance, even when it is not the relevant cue. Comparisons with symbolic and spatial cues show why the similarity between observed and executed actions matters. However, spatial correspondence must be varied separately from action identity: a faster response to a hand on the response side could otherwise be mislabelled imitation. The latency cost indicates competition or facilitation, not a complete account of voluntary copying or empathy.[ref]
Compatibility between observed and executed finger movements: comparing symbolic, spatial, and imitative cues by Marcel Brass and others. Abstract and Experiments 1–3, pp. 124–143: symbolic, spatial and imitative compatibility
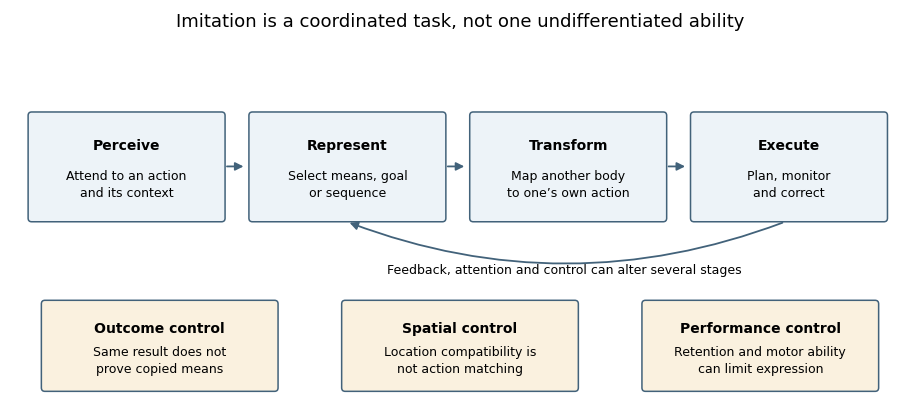
Psychological operations supporting imitation and their experimental controls
. Original functional schematic. The boxes identify task requirements and alternative explanations, not separate anatomical modules. Control and feedback can alter several stages. Details.
Control is as necessary as activation in many circumstances. A person may need to suppress the observed response and execute another instructed response, choose which part of a demonstration matters or adjust movement to a differently sized object. Attention determines which features are encoded; working memory supports sequences and deferred reproduction; motor planning and feedback determine whether an intended match is physically realized. A performance difference at any stage can reduce overt imitation, so failure does not uniquely show absence of a visuomotor mapping.
Goals can organize reproduction beyond visible movement. In a failed-action experiment, 18-month-old children often completed an adult’s intended target act even though the adult had not successfully demonstrated it. Control demonstrations and a mechanical-device comparison constrained accounts based simply on reproducing the visible trajectory. The result supports sensitivity to goal-directed human action, but completing the intended outcome is not proof of copying every bodily means or representing an explicit propositional belief. Goal inference and movement matching remain separable achievements.[ref]
Understanding the intentions of others: re-enactment of intended acts by 18-month-old children by Andrew N. Meltzoff. Experiments 1–2, pp. 838–850: failed attempts, completed acts and mechanical-device comparison
Infants’ copying can also vary with demonstration context. After seeing an adult activate a lamp using the head, 14-month-olds were more likely to repeat that means when the adult’s hands had been free than when the hands were occupied. One interpretation is that observers evaluate whether an unusual means was chosen freely or forced by a constraint. This motivates rational-imitation accounts. Yet differences in visible hands, attention or demonstration familiarity can also change encoding. Context sensitivity therefore requires explanation, but does not uniquely establish adult-like reasoning about reasons.[ref]
Rational imitation in preverbal infants by György Gergely and others. Abstract and p. 755: hands-free versus hands-occupied head-touch demonstration
Claims about prerequisites should also be developmentally precise. Neonatal matching, familiar automatic responses, newly learned gestures and extended technical procedures need not use identical representations or control demands. Disputed longitudinal neonatal findings emphasize the need for selective model-matching and appropriate control gestures rather than counting one commonly elicited action. Whatever their eventual interpretation, newborn findings do not license an inference that sophisticated intentional imitation is present at birth, nor does adult sensorimotor learning settle every neonatal result.[ref]
Comprehensive longitudinal study challenges the existence of neonatal imitation in humans by Janine Oostenbroek and others. Abstract: longitudinal tests across multiple modelled actions and early ages
The necessary psychological architecture is therefore a coordinated set of functions: detect relevant features, represent what is to be reproduced, transform that representation into feasible actions, retain it when required and control execution using feedback. Explicit intention understanding, social motivation and language can influence which actions are selected and why. They are not logical prerequisites for every compatibility effect. Good experiments manipulate these contributions separately and distinguish capacity from attention, opportunity and willingness to express it.
Interoception can contribute to social cognition by shaping emotional experience, the interpretation of others’ affect and the regulation of attention and action; it is not established as a universal prerequisite for understanding minds. Internal bodily signals are one source of information among visual, linguistic and contextual cues. A useful account must distinguish physiological state, detection of that state and interpretation of its significance.
Interoception includes processing signals related to the internal body. For social cognition, a faster heartbeat might contribute to experienced arousal, influence the significance of a threatening face or become evidence in an interpretation of one’s own discomfort during an interaction. The same change could accompany fear, effort or excitement. Bodily input therefore does not arrive with an unambiguous social label. Its contribution depends on context, expectations and the person’s ability to distinguish their own state from another’s.
Measurement is consequently central. Interoceptive accuracy is performance on an objective task; interoceptive sensibility concerns subjective reports; interoceptive awareness, in a more specific metacognitive framework, concerns how well confidence tracks actual performance. A primary comparison found these dimensions empirically dissociable rather than interchangeable. Someone who often attends to the body need not detect its signals accurately, and someone who performs accurately need not know when they are correct. A study connecting a questionnaire to empathy therefore cannot automatically be interpreted as connecting sensory accuracy to empathy.[ref]
Knowing your own heart: distinguishing interoceptive accuracy from interoceptive awareness by Sarah N. Garfinkel and others. Abstract and pp. 65–74: accuracy, sensibility and confidence–accuracy correspondence
Neuroimaging provides a plausible substrate. During heartbeat-timing judgments, right anterior insular/opercular activity related to objective performance, alongside a wider set of responses. This links a region involved in representing bodily state to measured interoceptive behaviour. Other work found affect-related insular recruitment when participants experienced pain themselves and when a partner experienced it. These observations support a possible bridge between self-state representation and vicarious affect, but anatomical overlap does not prove that exactly the same neurons or computations implement both functions.[ref]
Neural systems supporting interoceptive awareness by Hugo D. Critchley and others. Abstract and pp. 189–195: heartbeat-timing task, insular activity and performance
[ref]Empathy for pain involves the affective but not sensory components of pain by Tania Singer and others. Abstract: shared affect-related activity for self and partner pain
Manipulating when a social stimulus arrives offers a different test. A cardiac-phase experiment presented emotional faces at systole or diastole, using cardiac monitoring to time stimuli. Fearful faces were detected more easily and judged more intense at systole than diastole; associated imaging showed greater amygdala responses to fearful faces at systole. This shows that the bodily cycle can influence processing of an external affective cue even when the observer is not explicitly reasoning about their own heartbeat. It does not establish that consciously accurate heartbeat detection is necessary for the effect, or that cardiac phase explains every social judgment.[ref]
Fear from the heart: sensitivity to fear stimuli depends on individual heartbeats by Sarah N. Garfinkel and others. Abstract and Experiments 1–2, pp. 6573–6582: heartbeat-triggered faces, detection and intensity measures
Individual-difference evidence suggests another pathway. Alexithymia concerns identifying and describing one’s emotions, not having no emotions. In one study, empathy-related insula responses varied with alexithymia rather than autism diagnosis after adjustment. A separate psychophysical study associated alexithymia with interpreting facial expressions, while physical expression discrimination and identity judgments supplied important controls. Together they suggest that access to, or interpretation of, affective states may contribute to selected social-emotional tasks. They do not prove a single bodily-sensing deficit causes all these effects.[ref]
Empathic brain responses in insula are modulated by levels of alexithymia but not autism by Geoffrey Bird and others. Abstract: alexithymia and empathy-for-pain responses across diagnostic groups
[ref]Alexithymia, not autism, predicts poor recognition of emotional facial expressions by Richard Cook and others. Experiments 1–2: emotion attribution versus physical expression and identity discrimination
A direct interoceptive comparison also found that heartbeat-counting performance tracked alexithymia more clearly than autism across its tested groups. Its interpretation depends on the validity of the counting task. A common heartbeat counting score compares recorded counts and reported counts over intervals:A perfect heartbeat-counting score does not establish heartbeat detection: it only shows that reports matched recorded counts. Someone estimating from prior heart-rate knowledge can match the count without detecting individual beats. The score also depends mechanically on the denominator, so a relationship with actual heart rate needs interpretation. Empirical measurement analyses have exposed such problems; they qualify the inference from counting to perception, not the existence of bodily influences on cognition.[ref]
Alexithymia, not autism, is associated with impaired interoception by Punit Shah and others. Abstract and Experiments 1–2: alexithymia, autism and heartbeat-counting performance
[ref]Interoceptive accuracy scores from the heartbeat counting task are problematic: evidence from simple bivariate correlations by Giorgia Zamariola and others. Abstract and pp. 12–17: count-score relationships, actual heart rate and interval effects
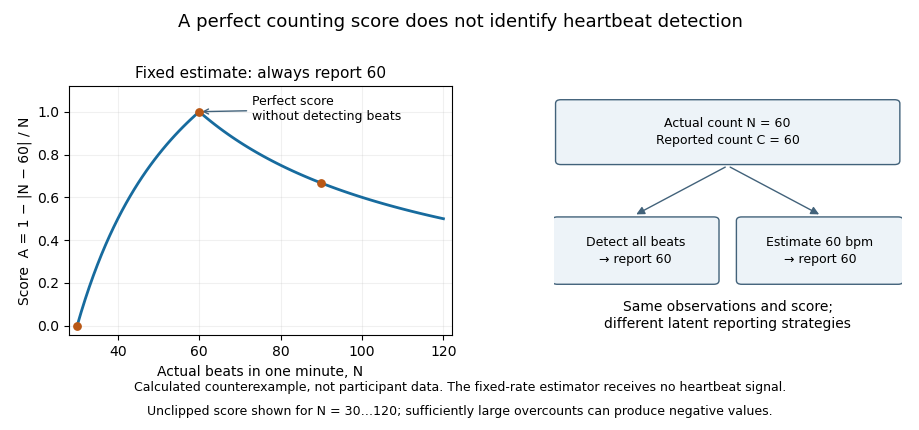

The statistical critique also needs qualification. A published reanalysis argued that several bivariate findings arise from analysing a ratio score and are less decisive than first claimed. This does not resolve every strategy or validity concern, and it does not invalidate the logical counterexample above. Mathematical dependence, sensory detection and behavioural usefulness should be tested as separate questions.[ref]
Are interoceptive accuracy scores from the heartbeat counting task problematic? A comment on Zamariola et al. (2018) by Daniel Zimprich and others. Abstract: reanalysis of ratio scores and qualifications to the bivariate criticisms
A strong interoceptive account must therefore specify the intermediate mechanism. Bodily input may change experienced affect, which changes attention to another person; uncertainty about one’s own state may complicate separating self-generated distress from another’s needs; physiological regulation may help sustain a demanding interaction. These are different causal routes. Each requires measurements of its proposed intermediate steps, temporal ordering and controls for general anxiety, task comprehension and sensory or motor demands. Merely correlating two questionnaires cannot choose among them.
There are also clear limits to generalization. Cardiac detection does not measure every visceral modality, and evidence about recognizing emotional faces does not automatically explain representing a false belief. A shared insular signal is not a complete theory of interpersonal understanding. Good tests combine validated bodily tasks, objective physiology, confidence measures and independently defined social outcomes, ideally manipulating bodily input while testing competing explanations. By the examination date, converging studies supported a contribution to some affective aspects of social cognition; the claim that one interoceptive deficit explains all social difficulties was substantially stronger than the evidence.
Atypical social cognition has helped decompose typical social functioning into separable perceptual, inferential, affective and control processes. Its greatest contribution is to reveal mechanisms and boundary conditions that a single average “social ability” score hides. It does not justify treating a diagnostic group as a simple subtraction of one module from an otherwise unchanged mind.
The general strategy resembles an experiment supplied by development or injury. If one function changes while another is relatively preserved, a single undifferentiated account becomes less plausible. But the inference depends on matching task demands, establishing a genuine dissociation and distinguishing acquired injury from lifelong developmental difference. Development reorganizes opportunities and learning across many years; a lesion can affect connected regions as well as local tissue. Neither is automatically a selective manipulation of a theoretical construct.
Focal amygdala damage illustrates how a seemingly emotional impairment can have a more specific perceptual mechanism. In a well-studied individual, difficulty recognizing fearful faces was linked to reduced spontaneous fixation of the eye region. Directing attention to the eyes improved recognition. This does not make the amygdala an isolated fear dictionary; it suggests a contribution to selecting diagnostic information. Typical emotion recognition must therefore include where information is sampled, not only how a fully inspected face is categorized. The case supplies a mechanistic hypothesis, with generality limited by its particular lesion and individual history.[ref]
A mechanism for impaired fear recognition after amygdala damage by Ralph Adolphs and others. Abstract and pp. 68–72: eye sampling, facial fear recognition and instruction
Lesion comparisons also help separate affective and cognitive contributions to empathy. Different inferior-frontal and ventromedial-prefrontal lesion patterns were associated with different emotional and cognitive empathy measures. This supports a multi-component view, provided task difficulty and lesion-network effects are considered. It is not evidence that every healthy person uses two wholly independent social modules. Rather, typical performance can combine distinguishable operations whose contributions become visible when one is disrupted.[ref]
Autistic participants have likewise challenged a global deficit account. A primary study found preserved performance on several goal-imitation and action-representation tasks alongside poorer theory-of-mind performance. Thus action matching, goal use and explicit mental-state inference should not be treated as equivalent tests. Typical social cognition also requires an account of how these processes interact, rather than assuming that a single observation–execution matching mechanism supplies them all. Behavioural preservation does not prove every neural circuit is unchanged.[ref]
Co-occurring characteristics can further change the inferred architecture. Empathy-related insula responses in one cross-group study tracked alexithymia rather than autism after adjustment. This suggests that affective and cognitive profiles can cut across diagnoses. The methodological lesson is to measure a candidate mechanism dimensionally instead of attributing every group difference to the diagnostic label. Adjustment is not an experimental manipulation, however: overlapping questionnaires, measurement error and selection can complicate interpretation, and correlation cannot establish which characteristic is causal.[ref]
Empathic brain responses in insula are modulated by levels of alexithymia but not autism by Geoffrey Bird and others. Abstract: dimensional alexithymia analysis across autistic and control groups
A selected psychopathy sample clarifies capacity versus spontaneous use. During uninstructed observation of emotional hand interactions, vicarious responses were reduced; when participants were explicitly asked to empathize, group differences were smaller. This suggests that the conditions recruiting a representation matter as well as whether it can be recruited. It does not establish identical processing throughout the brain or demonstrate normal everyday compassionate behaviour. Typical social cognition must therefore explain attention, motivation and instruction-dependent deployment alongside available representational capacity.[ref]
Reduced spontaneous but relatively normal deliberate vicarious representations in psychopathy by Harma Meffert and others. Abstract and observation-versus-instructed-empathy comparison, pp. 2550–2562
Interaction studies challenge the location of a difficulty. In story-transfer chains, autistic-only and non-autistic-only chains conveyed information more effectively than mixed chains under the tested conditions. Success depended on the pairing of communication partners, not simply on assigning each participant a fixed social score. This supports investigating shared conventions and interpersonal fit in typical interaction as well. It does not establish that every cross-neurotype interaction fails, that within-group communication is always effortless or that an information-transfer task captures every support need.[ref]
Autistic peer-to-peer information transfer is highly effective by Catherine J. Crompton and others. Abstract and Results, pp. 1704–1712: chain composition, information transfer and rapport
These findings improve theory only if the comparisons are well designed. Language, age, intellectual ability, sensory function and task familiarity may affect performance; matching one variable can inadvertently select unrepresentative groups. A group mean cannot classify every individual, and a nonsignificant difference is not proof of equality. Converging tasks should test the same hypothesized process, while discriminant measures check that it is not merely a general performance factor. Measurement invariance asks whether a score means the same thing across groups, rather than assuming identical interpretation of questionnaire items.
Causal conclusions also require triangulation. A focal lesion may support a necessary contribution to one task, an instruction manipulation can change deployment, and a correlational trait analysis can reveal heterogeneity. None alone establishes an entire developmental causal chain. Predictions should be tested in people without the original diagnosis or lesion where possible: for example, varying attention to facial features or explicitly separating mental-state inference from affect sharing. Such tests turn an atypical observation into a general model rather than an exceptional anecdote.
The resulting picture of typical social cognition is distributed, componential and relational. It depends on information sampling, learned representations, bodily affect, control and a partner’s responses. Atypical profiles have been informative precisely because they violate assumed equivalences among these functions. Their scientific value is greatest when individual variation is respected, findings are replicated across tasks and the explanatory target is a process in context rather than a claim that an entire group lacks social understanding.
The strongest explanation is a heterogeneous developmental account in which specific cognitive and sensory differences interact with co-occurring conditions and the social environment. No single deficit adequately explains all psychological difficulties experienced by autistic people. For particular emotional difficulties, alexithymia is a well-motivated candidate mechanism; for interpersonal difficulties, mismatched communication and exclusion are important competing or interacting causes. A useful explanation must say which outcome it explains and distinguish evidence from a broad label.
The outcome itself needs clarification. Differences in social communication, distress during unpredictable or sensory-demanding situations, difficulty identifying emotions and anxiety are not one psychological variable. An autistic person may show one without another, and outwardly similar avoidance can reflect different causes. Diagnostic criteria describe a pattern; they do not identify a single neural lesion, establish an absence of empathy or determine an individual’s quality of life. A theory should predict a specified process and explain variation within the autistic population as well as average differences from a comparison group.
A global theory-of-mind deficit is therefore insufficient. Mental-state reasoning can be difficult in some situations, and language, executive demands or spontaneous use can influence performance. Yet explicit task success and fluent conversation need not covary perfectly, while sensory overload and repetitive behaviour are not automatically consequences of failing a false-belief test. Calling every social misunderstanding mindblindness risks redescribing the outcome. The more precise question is which information the person represents, how it is accessed and whether the interaction supplies cues that both participants interpret similarly.
The broken-mirror hypothesis offers a neural mechanism but faces related specificity problems. One child study found preserved goal-imitation and action-representation measures despite differences in theory-of-mind performance. This challenges a universal failure of action matching as the cause of all autistic social difficulties. It does not prove every mirror-related response is typical; it shows why evidence about one imitation task or one activation contrast cannot stand for an entire diagnostic explanation. The developmental origin, current function and social consequences of a matching response require separate tests.[ref]
Imitation and action understanding in autistic spectrum disorders: how valid is the hypothesis of a deficit in the mirror neuron system? by Antonia Hamilton and others. Abstract: preserved action tasks, contrasting theory-of-mind performance and scope of the global mirror-deficit claim
Other single-process theories can contribute without becoming universal explanations. Differences in executive control may affect switching, planning or managing competing demands. Weak-central-coherence accounts emphasize local and contextual processing; social-motivation accounts emphasize orienting, reward and developmental experience. Predictive-processing accounts can formulate differences in expectations or the weight given to sensory evidence. Each needs independent measures and competing predictions. Observed withdrawal alone does not distinguish low social interest from anxiety, sensory strain or previous rejection, and a flexible account that explains any behaviour after the event is weak evidence for a mechanism.
For identifying emotions in oneself or others, alexithymia provides a more discriminating hypothesis. Across two psychophysical experiments, alexithymia related to difficulty interpreting emotional expressions, while controls separated expression interpretation from physical discrimination and identity judgments. An interoceptive study likewise associated its measured difficulty more clearly with alexithymia than autism. These results favour measuring a co-occurring dimension rather than treating emotional difficulty as a necessary feature of autism. They do not establish that every autistic person is alexithymic, or that alexithymia explains every communication or sensory difference.[ref]
Alexithymia, not autism, predicts poor recognition of emotional facial expressions by Richard Cook and others. Experiments 1–2: expression attribution, discrimination and identity controls
[ref]Alexithymia, not autism, is associated with impaired interoception by Punit Shah and others. Abstract and Experiments 1–2: alexithymia versus autism and heartbeat-counting performance
This account has testable limits. Alexithymia questionnaires require insight into one’s own emotional abilities, and heartbeat counting can be influenced by beliefs and timing strategies. Anxiety, language and overlapping questionnaire content may create or obscure associations. Consequently, converging behavioural, physiological and longitudinal measures are needed before inferring a causal chain from interoception through emotion identification to social difficulty. A selective association is useful evidence against diagnostic essentialism, but it is not a complete causal theory of autism.
A relational explanation addresses another level. The double-empathy proposal treats mutual understanding across differing experiences as a two-way problem. It was initially a theoretical argument, not proof that all difficulties are socially imposed. Experimental story-transfer work subsequently found that mixed-neurotype chains lost information more readily than same-neurotype chains in the tested setting. This is evidence that communication success depends on partner composition. It supports investigating shared expectations and conventions, while leaving open effects of familiarity, recruitment and the particular task.[ref]
On the ontological status of autism: the double empathy problem by Damian Milton. pp. 883–887: original reciprocity argument, distinguished from experimental evidence
[ref]Autistic peer-to-peer information transfer is highly effective by Catherine J. Crompton and others. Abstract and Results: mixed versus same-neurotype information-transfer chains
The wider environment can also contribute. In thin-slice studies, non-autistic observers formed less favourable first impressions of autistic speakers and expressed less willingness to interact; evaluating speech transcripts did not produce the same pattern as audiovisual presentation. Thus some barriers can arise from other people’s reactions to communication style rather than the substantive content conveyed. These controlled judgments do not establish the cause of every real-world relationship difficulty or later mental-health outcome. They nevertheless show why a theory confined to an autistic individual’s presumed deficit omits an experimentally demonstrated part of the interaction.[ref]
Neurotypical peers are less willing to interact with those with autism based on thin slice judgments by Noah J. Sasson and others. Abstract and Study 1: impression judgments, willingness to interact and transcript comparison
The most plausible explanatory programme combines these levels without treating them as interchangeable. A sensory or cognitive difference may change an interaction; repeated misunderstanding can alter expectations and anxiety; co-occurring emotion-identification difficulties may complicate recognizing or communicating distress. Those pathways are hypotheses to test prospectively, including autistic people with varied language and support needs. Results from verbally fluent research volunteers cannot represent the whole population, and support needs must not be dismissed merely because interpersonal context matters.
The decisive criterion is explanatory specificity. For a facial-emotion task, an alexithymia-related interpretation account can outperform a global autism-deficit explanation. For a difficult conversation, partner mismatch and exclusion may add explanatory power beyond an individual task score. For other outcomes, sensory, developmental or co-occurring clinical factors may dominate. This evidence favours multiple interacting mechanisms and individually measured needs over either a universal inability to understand minds or a claim that the social environment explains everything. It motivates scientifically testable, outcome-specific explanations rather than conclusions about an individual based solely on diagnosis.
Articles by others on the same topic
There are currently no matching articles.