Cytochrome P450s are versatile haem-containing oxidation enzymes that can install chemically difficult, highly selective functional groups. Photosynthetic microorganisms can supply their reducing equivalents and metabolic precursors, but useful production requires coordinated enzyme expression, electron delivery, substrate supply and product handling.
A Cytochrome P450 contains an iron–haem centre coordinated by a protein cysteine thiolate. The characteristic spectrum of its reduced carbon-monoxide complex gives the family its name. A common monooxygenation can be writtenOne oxygen atom enters the product and the other is reduced to water. Electron transfer and protonation activate bound oxygen, generating a powerful oxidant such as P450 compound I. Hydrogen abstraction followed by oxygen rebound can hydroxylate a C–H bond, but the family also supports other reactions, including epoxidation and successive oxidation steps. The exact chemistry is enzyme- and substrate-dependent; not every P450 simply performs a single hydroxylation.
This selectivity is valuable for complex natural products. Closely related substrates can differ in the position and stereochemistry of oxygenation, and an enzyme can distinguish sites that are difficult to separate by ordinary chemical synthesis. Oxygenated terpenoid intermediates, drug precursors and other specialized metabolites are therefore attractive targets. The opportunity is selective chemistry, not a guarantee that every plant pathway will be cheap to reproduce in a microbial host.
In an oxygenic photosynthetic chassis, light absorption by photosystem II supports extraction of electrons from water. Transfer through the photosynthetic chain and photosystem I generates reduced ferredoxin, which can feed a compatible P450 directly or contribute to NADPH production for an appropriate reductase system. The distinction matters: native microsomal P450s often use a flavoprotein reductase, whereas engineered direct ferredoxin delivery can bypass that partner. Electrons must still reach the P450 at adequate rates and with correct coupling to substrate oxidation.
There is a clear experimental proof of principle. A plant CYP79A1 catalytic domain was fused to the photosystem-associated PsaM anchor in a cyanobacterium, positioning it near the thylakoid electron supply. Activity was observed in light-driven experiments. This demonstrates functional rerouting of photosynthetic reducing power into a plant P450 reaction, rather than establishing commercial production of a finished pharmaceutical.[ref]
A production design starts from the entire pathway. Supply a suitable scaffold from endogenous metabolism or introduced enzymes, express the required P450s with compatible membrane anchors and redox partners, and include any downstream transferases or other finishing enzymes. CYP79A1, for example, participates in the pathway to dhurrin; expressing it alone establishes one activity, not the completed multienzyme pathway. For a new high-value oxygenated terpenoid, one must similarly verify every intermediate rather than equating scaffold accumulation with final-product synthesis.
Several constraints can dominate performance. Plant membrane enzymes may fold poorly, insert in the wrong orientation or fail to acquire haem. An abundant P450 may remain inactive because its substrate or electron donor is limiting. Competition with carbon fixation and essential redox metabolism can make maximal electron diversion harmful to growth. Uncoupled oxygen activation can generate reactive oxygen species instead of product. Excess light may increase oxidative damage, while high cell density limits light penetration. Oxygen supply is required for ordinary P450 monooxygenation even though the host produces oxygen photosynthetically.
Optimization should therefore measure carbon flux, enzyme abundance, redox state and products together. Adjust expression ratios, redox-partner choice, subcellular localization and induction timing; relieve precursor bottlenecks without starving essential pathways; and consider export or product capture to limit toxicity. A bioreactor must balance mixing, illuminated surface area, gas exchange and biomass density.
Useful controls include dark incubation, a catalytic-site mutant, pathway-minus strains and perturbation of photosynthetic electron supply while monitoring cell viability. Mass spectrometry and authentic standards establish product identity; oxygen uptake or a fluorescent reporter alone does not. Finally report titre, productivity, carbon yield and stability over repeated cultivation. Light-powered enzyme activity is the biochemical entry point; reliable, selective and economically recoverable product formation is the engineering goal.
Plant lipid diversity is generated by combinatorial biosynthesis in several compartments, selective exchange and remodeling, and evolutionary diversification of the underlying enzymes. Its functions extend from membrane mechanics and photosynthesis to storage, barriers and signaling, so no single adaptive explanation covers every lipid species.
At the simplest level, different acyl chains vary in length, double-bond number and position, and chemical substitution. Plastid fatty acid synthase builds chains carried by an acyl carrier protein. Chain termination and export determine which products enter further metabolism. Endoplasmic-reticulum fatty acid elongase enzymes extend selected acyl substrates, creating very-long-chain products used in surface and membrane lipids. Fatty acid desaturases introduce double bonds into particular substrates, while specialized enzyme variants can introduce hydroxyl groups or other unusual chemistry. Substrate specificity, reaction order and cellular location therefore generate many distinct acyl pools from a comparatively limited set of carbon precursors.
Chains are only one dimension. Acyltransferases assemble them onto glycerol or other backbones with positional specificity. Headgroup pathways generate glycerophospholipids and galactolipids, while distinct pathways produce sphingolipids and sterols. A lipid name such as phosphatidylcholine denotes a class, not a unique molecular species: two acyl chains can each vary, and their positions can matter. Storage triacylglycerols likewise combine many possible acyl groups. Functional diversity is therefore much larger than the number of lipid headgroups.
Compartmentation constrains which combinations occur. Plastid and ER assembly pathways use different enzymes and precursor pools, and products move between them. Monogalactosyldiacylglycerol and digalactosyldiacylglycerol are major constituents of photosynthetic membranes, whose requirements differ from those of the plasma membrane or a storage oil body. Acyl editing replaces chains on existing lipids, connecting synthesis to remodeling rather than simply producing a fixed end product. Selective transport, turnover and developmental expression create tissue-specific compositions even when the genome is unchanged.
An important test of functional importance comes from manipulating the enzymes rather than correlating lipid abundance with habitat. An Arabidopsis thaliana desaturase-deficient mutant lacking trienoic fatty acids was able to grow under permissive conditions but lost normal chloroplast performance during prolonged chilling. This supports a role for those acyl structures in maintaining photosynthetic function at low temperature.[ref]
Trienoic Fatty Acids Are Required to Maintain Chloroplast Function at Low Temperatures by Jean-Marc Routaboul and others. Desaturase-mutant physiology under low-temperature treatment
The inference is more precise than “unsaturated lipids are always better”: excessive unsaturation can also increase susceptibility to oxidation, and requirements depend on temperature and membrane function.Nutrient availability supplies another driver. Phospholipid synthesis requires phosphorus, whereas galactolipids can provide membrane material without a phosphate headgroup. Under phosphate deprivation, organelle lipid analyses detected redistribution of digalactosyldiacylglycerol into mitochondrial membranes. This demonstrates regulated compositional plasticity rather than requiring a new species to evolve every time phosphate becomes scarce.[ref]
Other selective pressures concern life on land and interactions with other organisms. Cutin, suberin and plant cuticular wax contribute to control of water loss, permeability and surface protection. Their chain lengths and oxygenation patterns affect packing and barrier properties. Seed oils store energy and carbon for establishment, while lipid-derived signals coordinate development and responses to damage. Pathogens, herbivores, drought, salinity and changing light environments can favour different combinations. A lipid useful as a defensive precursor may impose a cost on growth or oxidation resistance, creating trade-offs rather than one universal optimum.
Evolution can generate new chemistry through gene duplication, altered substrate specificity, changes in expression and retargeting of enzymes between compartments. A duplicated desaturase-like enzyme, for example, can retain the original reaction in one copy while another explores related substrate chemistry. Selection can preserve a useful product or tissue-specific role, while drift and biochemical side reactions also contribute to observed diversity. Cross-species lipid differences alone do not establish their adaptive value.
To separate these explanations, combine quantitative lipidomics, isotope tracing, enzyme biochemistry, genetic perturbation and physiological rescue. Compare plants at matched developmental stages and environments, because plastic remodeling can otherwise be mistaken for an evolved difference. The chemistry arises from modular enzymes and compartmentalized flux; the evolutionary explanation requires connecting particular molecular variants to performance in a defined ecological setting.
Both heterotrophic bacteria and oxygenic phototrophs must connect intracellular reducing power to an external acceptor across insulating cell-envelope layers. The best-characterized heterotrophic systems use dedicated respiratory redox conduits, whereas cyanobacterial export often involves mediators and incompletely resolved routes whose activity competes with photosynthetic metabolism.
In a Gram-negative heterotroph, oxidation of organic substrates supplies electrons to intracellular carriers and the inner-membrane quinone pool. An insoluble iron oxide or an electrode cannot enter the cytoplasm or simply accept an electron through the lipid phase. Extracellular electron transfer must bridge the inner membrane, periplasm and outer membrane before reaching the mineral or electrode surface. This is a sequence of chemically coupled steps, not unrestricted electronic conductivity through the whole cell.
Shewanella oneidensis provides a useful mechanistic example. Quinol oxidation connects through CymA and periplasmic carriers to the outer-membrane MtrCAB assembly. Its cytochromes place redox-active haem groups on the inward and outward sides of a porin-associated structure; surface MtrC can exchange electrons with external acceptors. Reconstitution of oriented MtrCAB in proteoliposomes demonstrated transfer from an internal electron-carrier pool to external Fe(III) oxides, directly testing the membrane-crossing function rather than inferring it from a mutant phenotype alone.[ref]
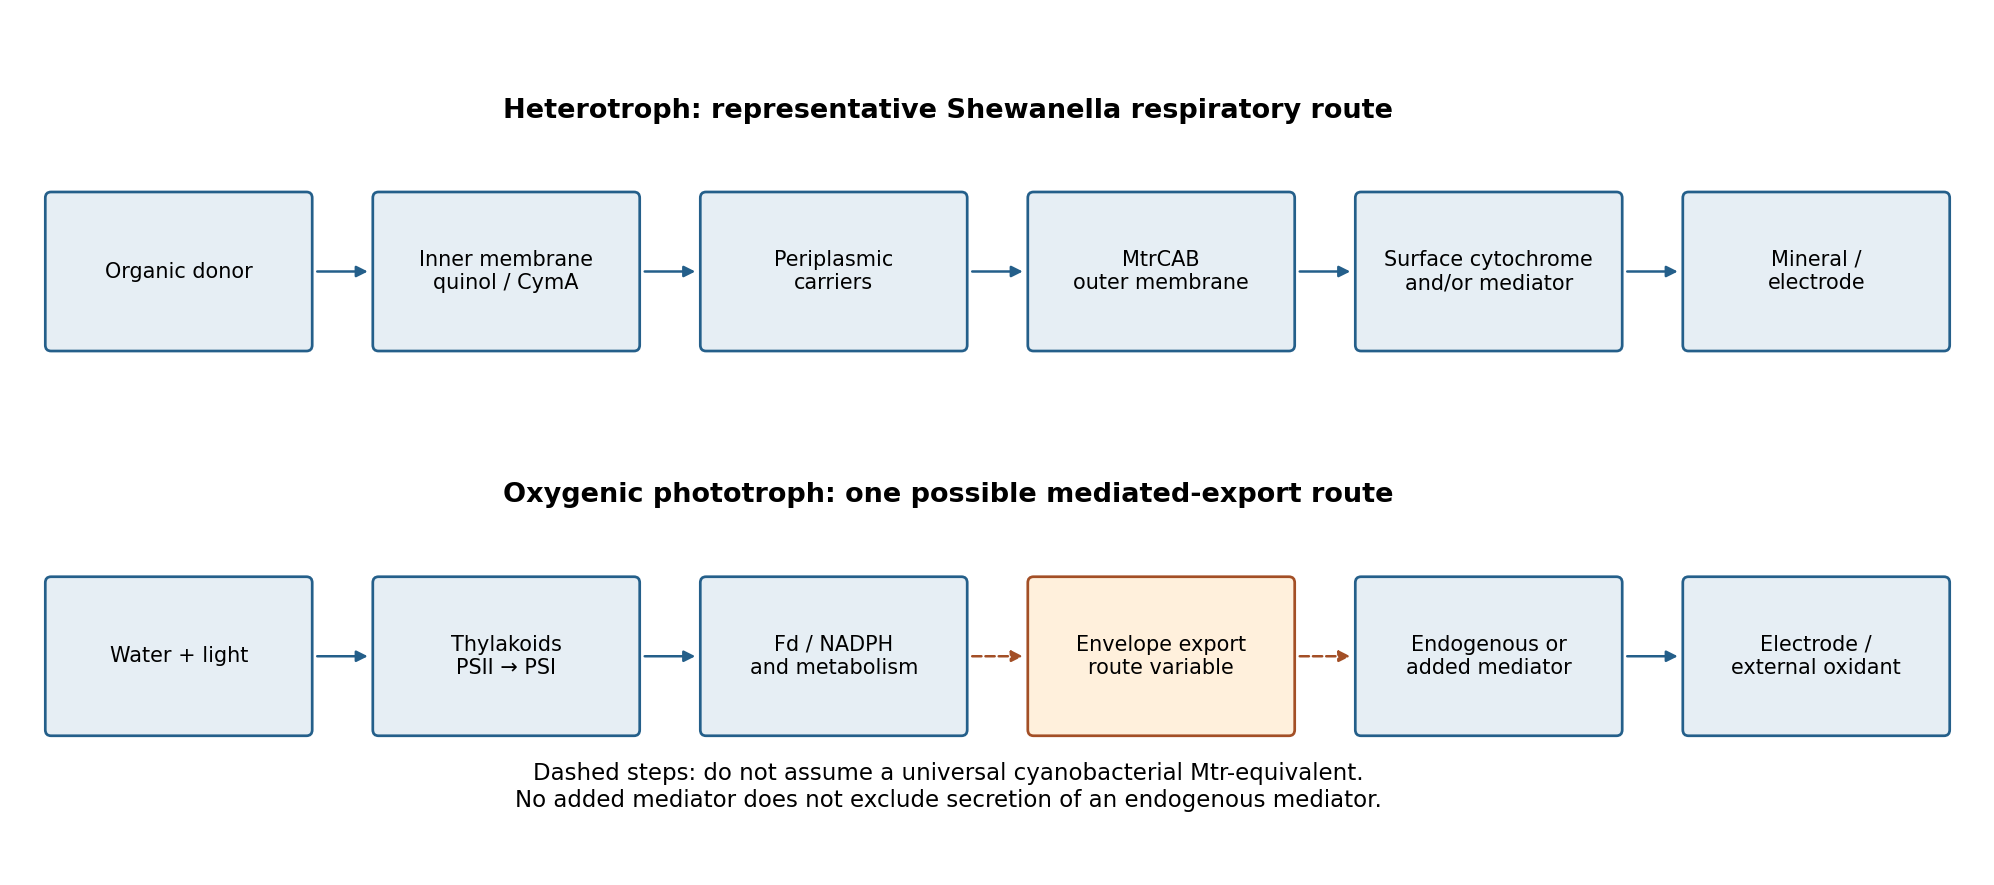
Original comparison of a characterized heterotrophic outer-membrane conduit with alternative phototrophic electron-export routes
. Details. 
Direct contact is one strategy. Surface cytochromes can reduce a mineral that is close enough, and extracellular conductive structures can extend electron transfer beyond the cell body. Some microbial nanowires are cytochrome-rich filaments or membrane-associated structures; the mechanism should be assigned to the organism and structure actually characterized. Calling every extracellular appendage a conducting pilus is unwarranted. Contact area, attachment and the conductivity of the surrounding biofilm can limit current even when the intracellular respiratory route is functional.
A second strategy uses a redox mediator. The cell reduces a soluble compound, which diffuses to a distant acceptor, transfers its electrons and returns in an oxidized form. Flavin-mediated transfer in Shewanella and phenazine-mediated transfer in some other bacteria illustrate how diffusible chemistry can complement direct contact. Some mediators also associate with proteins rather than remaining entirely free in solution. Mediator availability, diffusion, side reactions and loss into the environment therefore affect efficiency. A poised electrode and an insoluble mineral are not interchangeable acceptors: their accessible potentials, surface chemistry and spatial distribution differ.
For oxygenic phototrophs, light supplies a different upstream route. Photosystem II extracts electrons from water, and photosystem I generates reduced ferredoxin and downstream reducing power. In many cyanobacteria, these reactions occur on internal thylakoid membranes; an electron collected outside must therefore pass through additional metabolic and envelope steps. In eukaryotic algae, the chloroplast envelope and plasma membrane add further compartmental barriers. One should not transplant a Shewanella Mtr diagram into these organisms merely because both produce an electrode current.
The evidence for cyanobacterial export includes mediator-dependent reduction and sensitivity to envelope permeability. In one Synechocystis study, weakening outer-membrane attachment increased photocurrent, while replacing the culture supernatant with fresh medium removed that current under the tested conditions. Ferricyanide reduction provided a complementary readout. These results support a role for extracellular redox-active compounds and an envelope barrier, not identification of one universal cyanobacterial electron-export protein.[ref]
Order-of-magnitude enhancement in photocurrent generation of Synechocystis sp. PCC 6803 by outer membrane deprivation by Shoko Kusama and others. Outer-membrane perturbation, supernatant replacement and ferricyanide-reduction controls
The energetic roles also differ. Mineral-reducing heterotrophs can use an external acceptor in respiratory energy metabolism. A phototroph must retain enough reducing power for carbon fixation, nutrient assimilation and repair; maximal export is not automatically advantageous. Current can persist in darkness through metabolism of stored carbon, and secreted organic material can support heterotrophs that generate part of a measured community current. Oxygen evolution also changes local redox chemistry and can divert electrons away from the electrode.
Mechanistic experiments should separate these possibilities. Compare axenic cultures with mixed communities, light and dark conditions, intact and damaged cells, and cell-free supernatants. Use electrode-potential controls, viability assays, electron-transfer mutants and rescue, together with oxygen and carbon balances. Ferricyanide access must be interpreted relative to its membrane permeability. Most importantly, “no added mediator” does not prove direct transfer: cells can secrete their own mediator. The comparison is therefore between a relatively well-defined family of respiratory conduits and several phototrophic routes requiring organism-specific evidence, with the same general requirements of redox compatibility, envelope crossing and an accessible external sink.
Articles by others on the same topic
There are currently no matching articles.