Separate total methylated receptor from its active portion , where ligand-bound receptor is inactive and the unbound fraction supplies at finite ligand concentration. In the Barkai-Leibler model, receptor demethylation depends on the active portion:Every accessible stable steady state therefore obeysThe output is independent of chemoattractant even though the methylated pool changes. A ligand step first lowers , reducing its own reverse modification. Constant receptor methylation continues until recovers. Local stability follows from . This is output-dependent negative feedback. [ref]
Robustness in simple biochemical networks by Naama Barkai and Stanislas Leibler. 1997, model mechanism and adaptation precision
Changing CheR or CheB changes and the recovery time, but the return to each new pre-step baseline remains exact over the model's operating range. Robust perfect adaptation does not mean invariant tumbling frequency under changes in enzyme abundance. Nor does it extend to , or saturation of the finite receptor methylation capacity. If every receptor is permanently inactive, and the reverse flux cannot restore a positive baseline. The literal phrase that binding reduces activity to zero applies to bound receptors, not to every receptor under every finite stimulus.
If CheR instead follows Michaelis-Menten kinetics on unmethylated substrate, , thenAt steady state the forward flux becomes and generally depends on ligand through . Thus ligand-independent output is lost. Near-perfect adaptation can remain when so that CheR is effectively saturated, but Michaelis–Menten behavior outside that limit does not guarantee perfect adaptation. [ref]
Robust perfect adaptation in bacterial chemotaxis through integral feedback control by Tau-Mu Yi and others. 2000, analysis of ligand-independent bound CheR and the saturation assumption
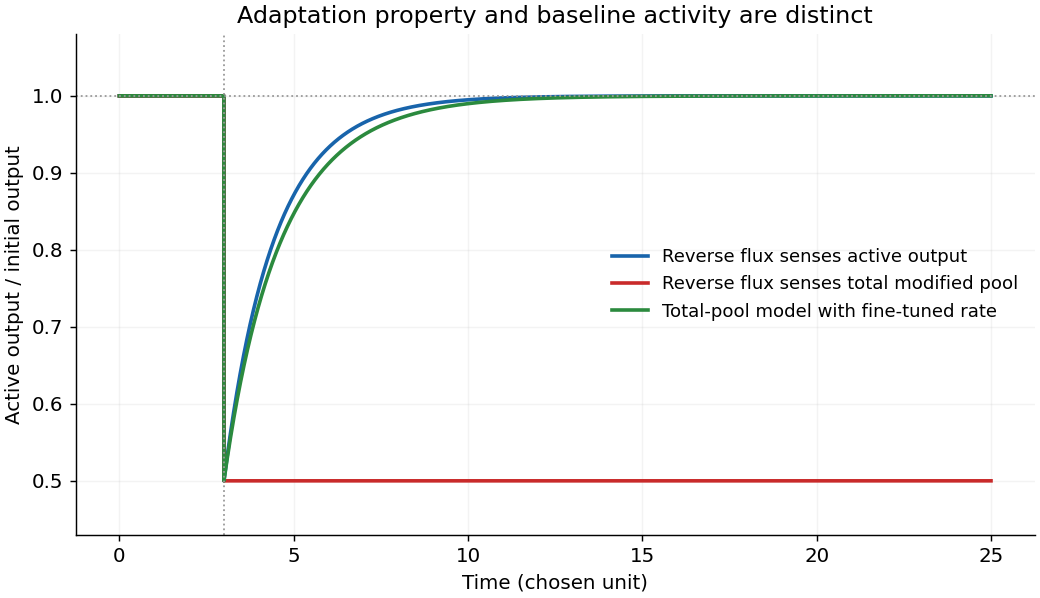
Fine tuning and output-dependent adaptation
. Original numerical solutions of the stated mathematical models. The ligand activity factor changes from one to one half; saturated output-dependent feedback restores activity, while a total-pool reverse reaction requires fine tuning. Details.
Articles by others on the same topic
There are currently no matching articles.