The bacterium samples its surroundings in time. A sustained increase in chemoattractant makes a favorable run persist by reducing the chance of tumbling; declining chemoattractant makes reorientation more likely. Individual tumbles need not point up the gradient. Biasing run durations can generate net migration even if reorientation itself is random. This is temporal comparison, not a direct measurement of a concentration gradient across the short cell body.
Compare the swimming time over length , , with diffusion over the same scale, . Their ratio is the Péclet number . The crossover estimate isOrder-one factors depend on the chosen diffusion-distance convention. A hypothetical stirrer of extent must instead have of order one, givingThese are transport-scale estimates, not a proof of a particular increase in uptake. Around a one-micrometre body, : local diffusive supply is already rapid. Actual uptake enhancement depends on the nutrient field and the cell's uptake boundary condition, neither supplied. The long run can help the organism reach a better nutrient region without implying that it greatly increases the flux from a uniform bath. E. coli normally uses bacterial flagella; the cilium in this comparison is a hypothetical generic stirring appendage, not its actual locomotor organelle.
Write , and . Saturated receptor methylation provides a constant positive flux, so the complete balance isAt a finite steady state, and thereforeThe derivative of the right side is , so this fixed point is stable in the scalar model. With total receptor concentration , it must additionally lie between zero and and leave sufficient substrate for the assumed saturated receptor methylation. If , the formal equation has no finite positive fixed point: finite receptor capacity then matters.
For an chemoattractant step, activity and hence tumbling frequency fall rapidly before receptor methylation can change appreciably. Slower chemical modification can then restore receptor signaling and make the tumbling frequency rise toward a new steady value. Perfect adaptation means return of that output to its original baseline despite the persistent chemoattractant step; it does not mean that receptor receptor methylation also returns to its original level.
The balance written here alone does not specify how ligand changes activity or receptor demethylation, and does not yet establish perfect adaptation. If activity is simply multiplied by a ligand-dependent fraction while this balance remains unchanged, is unchanged and the activity remains reduced. The following two models add different mechanisms that can compensate for that direct activity reduction.
Let chemoattractant reduce the activity per methylated receptor by a factor , with , taking the initial factor as one. The active output is . If changes to but receptor demethylation still acts on total methylated receptor, the new output isDemanding givesReduced receptor demethylation lets methylated receptors accumulate to , compensating exactly for their reduced activity. During the transition the activity first falls, then rises as receptor methylation accumulates. This compensation works only if the required methylated concentration is accessible; in particular in a finite receptor pool.
The required relation contains both enzyme concentrations. At fixed rates, increasing CheR raises the baseline receptor methylation and tumbling output, while increasing CheB lowers them. After such a change, the previous fine tuning generally no longer gives perfect adaptation. For example the required reverse capacity is , so changing without retuning changes the adapted output ratio. It is the precision of adaptation that is fragile here, in addition to the baseline itself changing. Changing all relevant capacities together in a way preserving the relation is a special exception, not generic robustness.
Separate total methylated receptor from its active portion , where ligand-bound receptor is inactive and the unbound fraction supplies at finite ligand concentration. In the Barkai-Leibler model, receptor demethylation depends on the active portion:Every accessible stable steady state therefore obeysThe output is independent of chemoattractant even though the methylated pool changes. A ligand step first lowers , reducing its own reverse modification. Constant receptor methylation continues until recovers. Local stability follows from . This is output-dependent negative feedback. [ref]
Robustness in simple biochemical networks by Naama Barkai and Stanislas Leibler. 1997, model mechanism and adaptation precision
Changing CheR or CheB changes and the recovery time, but the return to each new pre-step baseline remains exact over the model's operating range. Robust perfect adaptation does not mean invariant tumbling frequency under changes in enzyme abundance. Nor does it extend to , or saturation of the finite receptor methylation capacity. If every receptor is permanently inactive, and the reverse flux cannot restore a positive baseline. The literal phrase that binding reduces activity to zero applies to bound receptors, not to every receptor under every finite stimulus.
If CheR instead follows Michaelis-Menten kinetics on unmethylated substrate, , thenAt steady state the forward flux becomes and generally depends on ligand through . Thus ligand-independent output is lost. Near-perfect adaptation can remain when so that CheR is effectively saturated, but Michaelis–Menten behavior outside that limit does not guarantee perfect adaptation. [ref]
Robust perfect adaptation in bacterial chemotaxis through integral feedback control by Tau-Mu Yi and others. 2000, analysis of ligand-independent bound CheR and the saturation assumption
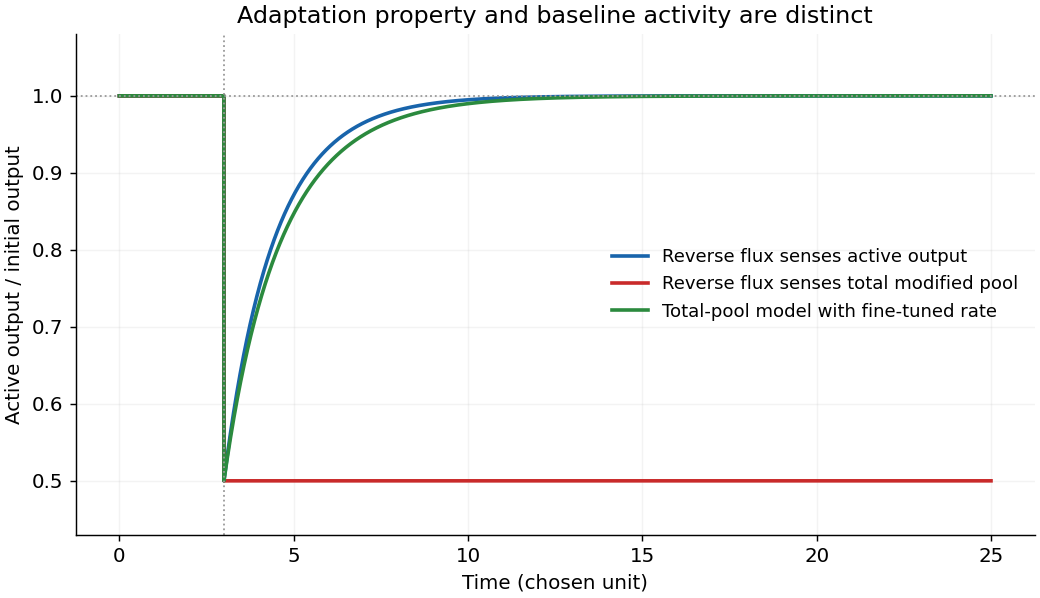
Fine tuning and output-dependent adaptation
. Original numerical solutions of the stated mathematical models. The ligand activity factor changes from one to one half; saturated output-dependent feedback restores activity, while a total-pool reverse reaction requires fine tuning. Details.
Articles by others on the same topic
There are currently no matching articles.