Original solutions to all six options in the Episodic and semantic memory course of the University of Oxford examination held on 3 June 2022. Question 1 retains its two printed Roman labels. The arguments use research available before the examination; the explanatory diagrams and counterexamples are original constructions.
Source: Oxford examination release, member a10975w1.pdf. The cover supplies the code and date; Part II is the frozen audited course classification.
Nonhuman animals retain information about particular past events, but this does not by itself establish human-like conscious recollection. The answer depends on what the category episodic memory requires. Knowing that an event happened differs from reliving it as something that happened to oneself. A species could possess useful event representations without satisfying every phenomenological criterion used in human research.
Endel Tulving's 1985 account makes autonoetic consciousness central: the rememberer apprehends the self in subjective time. This distinguishes episodic remembering from semantic memory, in which knowledge can be available without recollecting its acquisition. It is an influential theoretical proposal, supported by human observations and tasks, rather than an experiment establishing that every nonhuman species lacks that awareness.[ref]
Memory and consciousness by Endel Tulving. 1985, definitions of autonoetic awareness and distinctions among memory systems
The measurement problem is substantial. A verbal human report can distinguish knowing from remembering, although it is also vulnerable to instructions and interpretation. An animal's correct choice cannot supply the same report, and a failed verbal test would be inappropriate to its capacities. Thus absence of a linguistic demonstration is not evidence of absence of experience. Conversely, sophisticated behavior should not simply be renamed conscious reliving: trained rules, relative familiarity or a combination of independent cues may sometimes solve the task.
Converging evidence can narrow this uncertainty. Retaining a trial-specific combination, using it flexibly under an unexpected query, and distinguishing earlier from later events are stronger functional criteria than repeating a well-trained response. Hippocampal lesion effects that spare perception or simple item recognition further constrain the mechanism. Yet even a convincing functional resemblance does not uniquely decide whether subjective temporal self-awareness accompanies it. Anatomical similarity is supporting evidence about mechanisms, not a direct measure of private experience.
A defensible position therefore separates the phenomenon from the inference. If episodic memory is defined functionally as flexible memory for individual events and their relations, evidence from animals can support it. If the definition necessarily includes autonoetic consciousness, the same evidence leaves a further question unresolved. The available evidence supports substantial continuity in event-memory capacities, while remaining insufficient for an unqualified claim that animals consciously relive episodes in the human sense. That conclusion expresses a measurement limit rather than a claim that animal consciousness is impossible.
Evidence for episodic-like memory is substantially stronger, because its behavioral requirements can be tested without asserting conscious reliving. The strongest design establishes content, location and temporal information belonging to the same event, then shows that their combination guides behavior. Success on three unrelated tests would establish less.
Nicky Clayton and Anthony Dickinson's 1998 study exploited the ecology of food storage. Scrub jays cached perishable wax worms and nonperishable peanuts at distinct sites. They preferred recovering favored worms after a short interval, but learned to avoid searching for worms after a longer interval when those stores would have deteriorated. The choice therefore depended jointly on food type, caching location and delay, meeting a useful behavioral criterion for episodic-like memory.[ref]
Episodic-like memory during cache recovery by scrub jays by Nicky Clayton and others. 1998, cache contents, spatially distinct sites and interval-dependent recovery
This result should not be expanded into a claim of complete freedom from learned knowledge. Knowledge that worms deteriorate supplies an enduring rule about food, while memory of a particular cache supplies event-specific input to the rule. An episodic-like account can therefore require interaction with learned knowledge rather than its absence. Critical controls and extensions should remove immediately informative odor cues, separate elapsed time from time of day, counterbalance item preferences, and test combinations that cannot be answered by one permanently rewarded location. Such controls are requirements for discriminating explanations, not additional findings attributed here to the original paper.
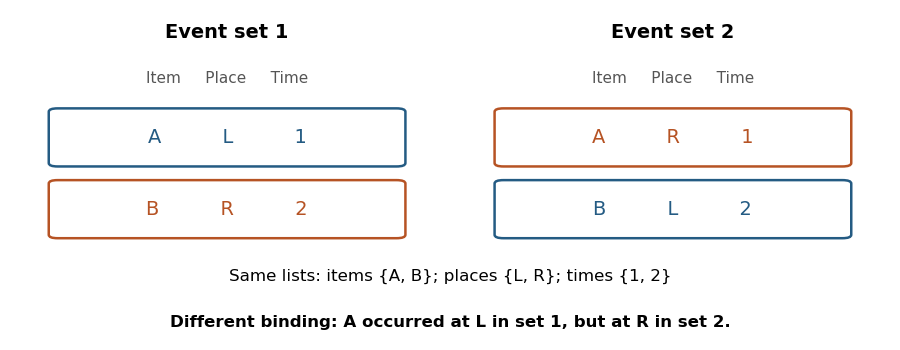
An original example illustrates why conjunction matters. Compare the two event setsBoth contain the same items, places and temporal positions. However, the correct answer to where occurred differs. Separate lists cannot determine that answer. Episodic binding is therefore a stronger claim than retaining the three lists, and a useful experiment tests a relation whose answer changes across otherwise matched combinations.
Rodent studies provide complementary causal evidence. Norbert J. Fortin and colleagues found impaired memory for the order of odor events after hippocampal lesions despite preserved recognition of recently presented odors. Ceren Ergorul and colleagues presented odor events at different locations and found that intact rats used combinations of odor and spatial cues in temporal judgments, whereas hippocampal lesions disrupted this integration. Their probe tests help distinguish a binding deficit from simply being unable to detect the individual cues.[ref]
Critical role of the hippocampus in memory for sequences of events by Norbert J. Fortin and others. 2002, sequence-order versus item-recognition comparison
[ref]The hippocampus and memory for what, where, and when by Ceren Ergorul and others. 2004, single episodes and cue-combination probes
These studies support event-specific relational retention across different species and tasks. They leave open how much a given test depends on relative recency, familiarity or a learned retrieval strategy; selective transfer and matched recognition controls are particularly useful. Episodic-like memory is supported as a graded collection of experimentally demonstrated capacities, without treating every such success as proof of autonoetic remembering.
Content, space and time show partly different neural emphases, but their conjunction is distributed across interacting populations rather than stored in three independent boxes. The same experimental result can concern sensory selectivity, encoding, retention or retrieval. Distinguishing these stages prevents an area that responds to a stimulus from being identified automatically as the permanent store of its memory.
For item information, the perirhinal cortex is a useful starting point. Its connections and representational properties make it important for distinguishing complex objects and their familiarity. Lila Davachi and colleagues in 2003 used event-related functional magnetic resonance imaging while participants encoded adjectives through scene imagery or a reading transformation. Later tests separated item recognition from remembering the encoding source. Perirhinal encoding activity predicted later item recognition; hippocampal and posterior parahippocampal encoding activity predicted source recollection. This supports distinguishable contributions, not a proof that the hippocampus never represents an item or that perirhinal activity cannot depend on context.[ref]
Multiple routes to memory by Lila Davachi and others. 2003, encoding tasks and subsequent item/source memory effects
Spatial information is likewise heterogeneous. A place cell is selective for the animal's location under specified conditions, whereas a spatial view cell concerns a viewed location. The distinction matters in primates, where gaze and bodily position can vary independently. Recordings associated with Edmund T. Rolls tracked viewing and movement to distinguish spatial-view responses from self-location. Such cells establish an available code for a spatial variable; they do not demonstrate that the code alone contains an entire episode.[ref]
Spatial view cells in the primate hippocampus by Edmund T. Rolls and others. 1997, active locomotion, eye-position controls and allocentric viewed location
The parahippocampal cortex, entorhinal cortex and hippocampus participate in contextual and spatial processing, with reciprocal cortical interactions. A scene or context can help specify where an item belongs, while an item's identity can change the significance of a location. Thus “what” and “where” are distinguishable questions without requiring completely independent neuronal populations. A location-selective cell may also depend on the task, preceding event or remembered destination.
Temporal information requires a further distinction between elapsed duration, relative order and a date-like temporal context. Norbert J. Fortin's odor-order result shows that hippocampal dependence is not confined to spatial arrangements: remembering a nonspatial sequence can be impaired even when recent-item recognition remains possible. However, an earlier-versus-later judgment need not use an explicit clock. A change in trace strength can sometimes serve as a recency cue, so order and recognition controls are essential.[ref]
Critical role of the hippocampus in memory for sequences of events by Norbert J. Fortin and others. 2002, nonspatial sequence task and recognition control
Christopher J. MacDonald and colleagues' 2011 recordings provide a cellular example. Rats performed object–delay–odor sequences, requiring the earlier object to guide the later odor response. Successive hippocampal cells were active at different parts of the intervening interval; changing its duration caused many cells to alter their temporal organization. These time cells could also carry location, behavior or sequence information. The result is more consistent with temporally organized population states than with every neuron being assigned exclusively to one content dimension.[ref]
Hippocampal time cells bridge the gap in memory for discontiguous events by Christopher J. MacDonald and others. 2011, object–delay–odor task, interval responses and retiming
The coding similarities are therefore as informative as the differences. Spatial and temporal selectivity can both form sequences of changing activity; either can be combined with an object's identity. Mixed selectivity permits a representation to distinguish the same item in different contexts. An analysis should vary content, place and timing independently wherever possible, because locomotion, expectation, reward and elapsed time are often correlated. Decoding a variable from correlated neural data shows available information, not necessarily a dedicated code for that variable.
Finally, retrieving a particular conjunction differs from retaining isolated features. The counterexample of identical marginal lists with different bindings demonstrates this logically. Neural evidence should therefore test whether a pattern distinguishes the correct relations, generalizes to a new query, and predicts errors that specifically confuse bindings. Single-cell recordings provide timing and selectivity; imaging samples wider regions; lesions test necessity under particular task conditions. Each method addresses a different part of the claim.
The best account is differentiated inputs and computations combined into event representations, with content, place and time often expressed jointly. Neither regional specialization nor mixed coding eliminates the need to explain how the correct features are bound and later accessed.
Specific memory operations can depend on communication between regions even when the required information is measurable within each region separately. Binding an event, selecting its relevant context and using it to guide a response impose different demands. Regional involvement alone does not tell us whether two regions cooperate, act in parallel or merely share an input. Two experimentally characterized interactions illustrate what stronger evidence can establish.
For hippocampal–prefrontal coordination, Matthew W. Jones and Matthew A. Wilson in 2005 recorded simultaneously with tetrodes in rat hippocampal CA1 and medial prefrontal cortex during a spatial memory task. Correlated firing and coupling in the theta range increased during behavior recruiting spatial working memory. This links interaction to a particular task demand rather than merely showing that both areas are active. It offers a mechanism by which spatial information can become coordinated with task-dependent behavior.[ref]
Theta rhythms coordinate hippocampal-prefrontal interactions in a spatial memory task by Matthew W. Jones and others. 2005, simultaneous CA1/PFC recordings, correlated firing and task-selective theta coupling
The proposed benefit of timing is precise: if downstream neurons are sensitive to when inputs arrive, consistent relative phases can make selected inputs effective together. This does not mean that synchrony itself supplies the remembered content. Nor does a common theta rhythm prove transmission from one named region to the other. Shared rhythmic input, changes in movement or another task-related state could increase coupling. Correlation provides evidence for functional connectivity; demonstrating the necessary route or direction requires a stronger intervention or a constrained causal model.
The hippocampal–retrosplenial example adds such an intervention. Brenton G. Cooper and colleagues in 2001 combined temporary retrosplenial cortex inactivation with hippocampal recordings during radial-maze behavior. Place-field locations changed during inactivation. In well-trained animals, behavioral impairment was particularly evident in darkness, when visual landmarks could not supply the same information. Crucially, changes in hippocampal spatial coding also occurred without a behavioral deficit in other conditions. Remote neural reorganization and overt impairment therefore need not have a one-to-one relation.[ref]
Temporary inactivation of the retrosplenial cortex causes a transient reorganization of spatial coding in the hippocampus by Brenton G. Cooper and others. 2001, Experiments 1–2, light/dark conditions and hippocampal coding changes
This finding supports a causal dependence of hippocampal coding on the state of retrosplenial circuitry. A plausible interpretation is that the network combines landmark and movement-related information to maintain spatial context. It remains an interpretation of the computation, not proof of a direct monosynaptic message or a complete model of human recollection. Inactivation can influence indirect pathways, and a spatial navigation task tests ingredients useful for episodes without itself demonstrating autonoetic recall.
These interactions can be related to specific mnemonic demands. A hippocampal representation may distinguish the relationships within an event, while a prefrontal interaction makes the appropriate relationship relevant to the current rule or query. A retrosplenial interaction may help maintain or update the spatial frame in which that relationship is interpreted. The hypotheses predict different vulnerabilities: changing retrieval goals should particularly challenge selection, whereas removing reliable external spatial cues should increase reliance on internally updated context. They do not require every region, including all posterior parietal subdivisions, to be equally necessary on every trial.
A particularly informative next experiment would combine a controlled perturbation with simultaneous recording and a task that dissociates item recognition, spatial binding and source or sequence judgments. Preserved recognition alongside disrupted binding would narrow a general arousal or sensory explanation. Comparing matched movement and reward conditions would test behavioral confounds. A crossed disconnection experiment could examine cooperation between a specified pair if the relevant pathways and their laterality were established: the comparison must include unilateral and same-side controls rather than assuming that any two lesions diagnose an interaction.
The critical question is not simply whether performance declines. The perturbation should disrupt the predicted representation or its task-dependent use at the relevant time, and the remote change should be measured. Even this requires caution about indirect effects and compensation. Conversely, normal performance after perturbation may reflect redundant routes or the availability of external cues, rather than complete irrelevance of the region.
The evidence supports task-dependent interactions for coordinating, contextualizing and using event information. It does not justify equating a regional activation map, a synchrony measure or one navigation impairment with a universal four-region circuit for every aspect of episodic remembering.
The theories can be reconciled at several explanatory levels, but a strong restriction of medial temporal regions to declarative memory conflicts with evidence for their contribution to demanding online perception. Compatibility should be assessed between explicit claims, rather than achieved by renaming every deficit relational or mnemonic.
The medial temporal lobe declarative memory system theory, associated with Larry Squire and Stuart Zola-Morgan, identifies a system important for rapidly establishing long-term memories for facts and events. Their 1991 account emphasizes binding distributed cortical representations and a time-limited dependence during consolidation. It explains why substantial impairment in acquiring new declarative knowledge can coexist with preserved skills or other learning. The proposal specifies a memory system and its temporal role; it does not by itself specify every representation or learning rule inside each component.[ref]
The medial temporal lobe memory system by Larry Squire and others. 1991, anatomical components, declarative learning, cortical binding and consolidation
Relational memory theory, associated with Howard Eichenbaum and supported by work including Norbert J. Fortin's, addresses the organization and flexible use of relationships. Items may be connected by location, order or another shared element. The account therefore explains why hippocampal damage can affect more than a spatial map. Its proposal that related experiences support flexible queries supplies a candidate computation within a wider declarative system, rather than necessarily competing with the existence of that system.[ref]
The hippocampus and mechanisms of declarative memory by Howard Eichenbaum. 1999, systematic organization and flexible expression of memories
The representational hierarchy theory associated with Timothy J. Bussey and Mark J. Buckley asks what conjunctions a region represents. A simple feature can occur in several objects and be insufficient for distinguishing them. Perirhinal object-level representations can reduce such ambiguity. The same representation can support recognizing an object after a delay or distinguishing it among simultaneously visible alternatives; the representational demand crosses the usual perception–memory boundary.
Two experiments sharpen this claim. Timothy J. Bussey and colleagues in 2002 held the number of object pairs constant while varying feature ambiguity in visual discrimination. Perirhinal lesion effects were related to the conjunction demand, supporting a more specific account than simply more objects or more difficult learning. Mark J. Buckley and colleagues in 2001 used simultaneous touchscreen oddity tasks. Lesioned macaques were impaired when object-level distinctions were required, with spared performance on difficult discriminations based on simple color, shape or size differences. Difficulty alone therefore does not explain the pattern.[ref]
Perirhinal cortex resolves feature ambiguity in complex visual discriminations by Timothy J. Bussey and others. 2002, fixed number of pairs and manipulated feature ambiguity
[ref]Selective perceptual impairments after perirhinal cortex ablation by Mark J. Buckley and others. 2001, object oddity and difficult simple-feature controls
A constructive reconciliation follows. The declarative account identifies a broad system and its role in long-term learning; the relational account specifies organization and flexible expression; a representational hierarchy specifies which conjunctions its components can supply. Perirhinal object representations and contextual representations can participate in hippocampal binding, and learning can stabilize those relations. Item/source differences in Lila Davachi's encoding study are consistent with differentiated contributions within a common system. Consistency is weaker than a unique confirmation of this particular synthesis.[ref]
Multiple routes to memory by Lila Davachi and others. 2003, differentiated subsequent item and source memory effects
A real disagreement remains. If an original strong declarative-only position says that these regions have no necessary role in perception or immediate processing, a selective deficit on simultaneous object discrimination is problematic. Calling every across-fixation comparison memory would protect that position only by changing what it excludes. Conversely, simultaneous display does not eliminate working memory, attention, task-rule learning or all incidental encoding. The strongest adjudication manipulates representational complexity separately from retention demand and matches sensory and motor requirements. A selective conjunction deficit at negligible imposed delay supports the representational claim more directly than a generic difficult-task impairment.
The theories also need not agree about eventual hippocampal independence of detailed remote episodes. Systems-level consolidation, relational organization and perceptual conjunctions are different issues; adopting one does not logically settle the others. Each retained commitment should generate a prediction that could differ from an alternative, including the kind of error expected after a selective lesion.
A coherent account can combine a differentiated medial temporal system, relational binding and hierarchical representations. It must explicitly revise a strict memory-only boundary if complex online perception requires the same representations; that tension cannot be removed merely by saying that all three theories describe different levels.
Episodes can be encoded through learned relationships among distributed neuronal activity patterns, with temporal context distinguishing successive events and selective reinstatement supporting retrieval. A satisfactory explanation needs more than a neuron that responds during an experience. It must account for persistence after the event, separation of similar events and access from a partial cue.
At encoding, different populations carry information about content, context, actions and internal state. A cell assembly can represent their conjunction through coordinated activity rather than assigning one exclusive neuron to each episode. Mixed selectivity permits the same cell to contribute differently when an item occurs in different contexts. Synaptic plasticity can preserve changes in interactions after the original activity stops. Thus remembering need not require the encoding neurons to fire continuously throughout retention.
A simplified Hebbian learning rule makes the proposal concrete. If two activities are and , an update , with , strengthens their association under the model. Recurrent interactions can later support pattern completion from a partial cue, while pattern separation can reduce confusion between similar inputs. These operations fit the anatomy of hippocampal circuits, but the equation is an idealized storage rule, not a complete experimentally established biochemical mechanism. Stability, interference and correct downstream readout remain additional requirements.
Order creates a further constraint. Suppose a putative episode is stored only throughReversing the order of the vectors leaves the sum unchanged. Such an order-insensitive update cannot distinguish the original sequence from its reversal. Temporal context, directed transition learning or trace learning must add information if order matters. This is a mathematical limitation of the displayed rule, not evidence that all Hebbian mechanisms lack temporal sensitivity.
Christopher J. MacDonald's time-cell findings supply a candidate representational ingredient: population activity changes across an interval and can depend on which event initiated the sequence. An item can therefore become linked to a changing state rather than to a timeless list. Because cells also encode behavior and location, experimental controls must separate elapsed time from correlated actions or expectations. The repeated trained sequence demonstrates an available temporal coding mechanism, not a recording of every feature of a unique autobiographical episode.[ref]
Hippocampal time cells bridge the gap in memory for discontiguous events by Christopher J. MacDonald and others. 2011, delay coding and sequence-dependent responses
Retrieval offers another test. Hagar Gelbard-Sagiv and colleagues in 2008 recorded single neurons in human hippocampal and nearby regions while patients watched cinematic episodes and later freely recalled them. Selective reactivation of some of the same hippocampal and entorhinal neurons preceded verbal recall of the corresponding episode. This connects internally generated activity with specific remembered content. It does not establish that one cell contains the entire memory, that every encoded cell must reactivate, or that the recorded activity causes the subjective experience.[ref]
Internally generated reactivation of single neurons in human hippocampus during free recall by Hagar Gelbard-Sagiv and others. 2008, cinematic episodes, free verbal recall and selective cellular reactivation
Causal work addresses a different level. Tomás J. Ryan and colleagues in 2015 tagged learning-associated cell ensembles in mice. Artificial activation could elicit memory-related fear behavior even under experimentally induced amnesia. This supports a distinction between failure of natural access and complete loss of every retained trace. Artificially evoked freezing is nevertheless a behavioral readout; it does not demonstrate recovery of all episode details or autonoetic consciousness. Appropriate control ensembles and contexts are needed to distinguish selective access from nonspecific recruitment of defensive behavior.[ref]
Engram cells retain memory under retrograde amnesia by Tomás J. Ryan and others. 2015, tagged ensembles, amnesia and artificially evoked memory behavior
These findings motivate an interacting account of storage and retrieval. Distributed representations supply content; learned connections bind and separate events; evolving activity supplies temporal position; a retrieval cue recruits an appropriate pattern. Reinstatement can be partial and transformed by the current goal, rather than a literal replay of every original sensory input. Semantic memory can provide the enduring knowledge used to interpret an episode without replacing its event-specific relations.
The strongest explanation combines population representations, persistent plastic changes, temporal organization and selective retrieval. Recording selectivity, identifying an engram and showing behavior after stimulation are complementary findings; none alone amounts to a complete neural account of an experienced episode.
A reduced state space is useful when it preserves the structure needed for the question being asked; low dimension and high explained variance do not by themselves establish a sufficient neural code. Start with a clear observation model. A vector of binned spike counts from neurons may be approximated through latent coordinates, but the choices of bins, transformations, noise model and preserved criterion all affect the result.
For centered observations, principal component analysis chooses an orthonormal projection to minimize expected squared reconstruction error,where . The identity follows by expanding the square and using . Diagonalize . The trace term is , with for the columns of . Here and because the columns of are orthonormal. Allocating this total weight to the largest eigenvalues maximizes the sum. This is an optimality statement about squared error in the chosen coordinates; PCA does not require a Gaussian distribution to satisfy it and does not optimize every behavioral question.
An exact counterexample makes the limitation decisive. Let be independent balanced signs, define , and let the remembered class be . Zero means and independence giveThe first component retains of total variance. Yet : no classifier using that component alone exceeds one-half expected accuracy. The second component determines the class exactly. Positive rates give the same example after centering. These are constructed rates, not experimental recordings.
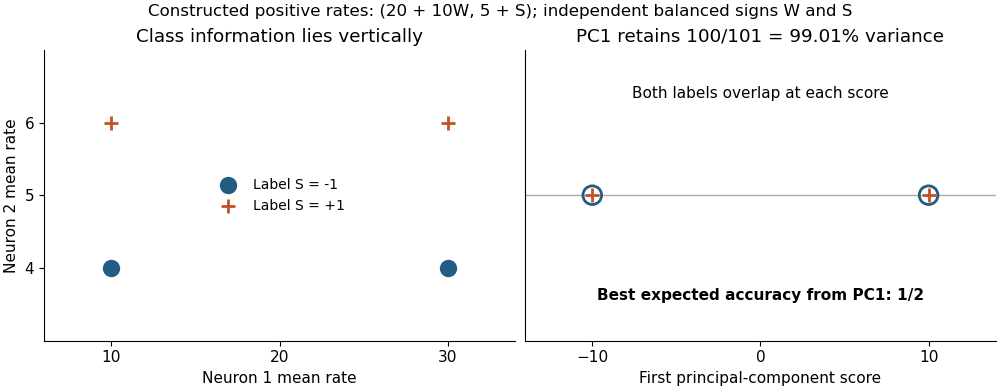


This example also exposes a scaling assumption. Covariance-based PCA emphasizes large-variance coordinates; standardization changes that objective and may increase the influence of noisy low-rate cells. Neither preprocessing choice is automatically correct. Behaviorally relevant information may lie in a small-amplitude direction, in precise spike timing lost by binning, or in correlations not retained by a rate-only summary. Dimensionality must therefore be evaluated against decoding, reconstruction and the scientific question separately.
Byron M. Yu and colleagues' 2009 Gaussian-process factor analysis combined temporal smoothing and dimensionality reduction in a probabilistic framework. Its demonstration used 61 simultaneously recorded macaque premotor and motor neurons during reaching. It shows a method for estimating single-trial trajectories, not direct evidence that episodic memories have the same dimensional structure.[ref]
Gaussian-process factor analysis for low-dimensional single-trial analysis of neural population activity by Byron M. Yu and others. 2009, observation model, temporal priors and motor-recording demonstration
In a linear observation model , the noise and latent temporal assumptions matter. A Gaussian observation approximation can be imperfect for sparse counts; independent residual errors can misassign shared fluctuations; a smooth temporal prior can suppress abrupt transitions. Trial averaging can manufacture a smooth path while concealing different single-trial paths. A useful low-dimensional description must also generalize beyond the sampled cells, session and task: unrecorded populations may encode variables absent from the fitted coordinates.
Latent axes require care as well. In , an orthogonal rotation gives the identical reconstruction through and , because . Reconstruction alone therefore cannot label one axis a unique psychological process. Model priors and constraints can restrict this ambiguity. Similarly, attractive geometry does not establish intrinsic dynamics: unobserved inputs, behavior or the analysis itself may shape the apparent trajectory. If a true dynamical state is claimed, the retained coordinates should predict relevant future activity under a specified model, not merely provide a convenient picture.
Validation should choose dimension and preprocessing within training data, then assess held-out trials or sessions and, where appropriate, held-out neurons. Behavioral labels must be kept out of unsupervised fitting decisions used to claim independent prediction. Comparing multiple dimensions and reporting uncertainty is more informative than selecting the most compelling two-dimensional plot. A reduced representation can support a useful decoder without being a complete causal explanation of the circuit.
Low-dimensional state spaces are testable approximations whose value depends on retained information, model fit and generalization. The projection, scaling, temporal and sampling assumptions should remain explicit, especially when a high-variance view is being interpreted as the mechanism of episodic memory.
Articles by others on the same topic
There are currently no matching articles.