Signal amplification is an increase in a specified downstream response relative to an initiating signal. In a molecular-count description, one activated component can generate or activate many downstream molecules. Repeated catalysis by an enzyme supplies a mechanism: the enzyme remains available for another chemical reaction. Successive stages can multiply the response. For a biological example, Cooper describes the epinephrine-to-glycogen phosphorylase pathway, where production of many cAMP molecules and repeated downstream protein phosphorylation provide opportunities for signal amplification. This is an example, not a claim that every signal transduction pathway has the same stages or gain. [ref]
Here is a counting toy extending the example under signal transduction. Suppose activated receptors each activate distinct relay proteins during a first interval. During a subsequent interval, each relay activates distinct target proteins. Assume enough inactive relays and targets, no shared targets, and no loss of activity during the count. ThenFor , this gives and : the target-to-receptor count ratio is . These are assumed integer counts, not measured rates or a universal physiological amplification factor. The intervals are sequential; the equations do not specify a time course.
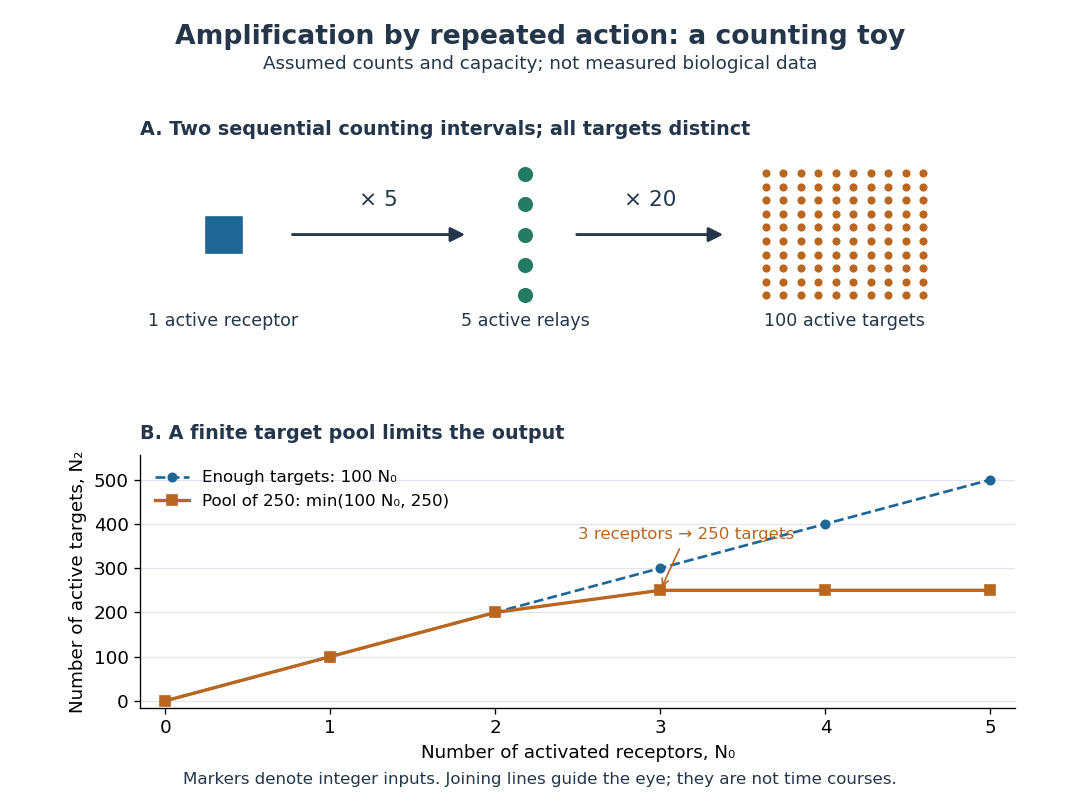

Availability limits the multiplication. As a second toy assumption, let there be only initially inactive target proteins shared by all branches, and suppose the branches can activate distinct targets until this pool is exhausted. ThenTwo activated receptors give active targets, whereas three give , not . At three activated receptors, the total count ratio is ; adding a fourth activates no additional targets. Thus total output per input and the increment caused by an extra input are different notions of gain. This finite-pool rule is an illustrative bound, not an enzyme kinetics law.
Signal amplification makes a small initiating signal capable of a larger response, but it does not supply the material or energy for downstream chemical reactions. In the second messenger transfer experiment, both stages still required added ATP and magnesium ions. Counts, changes in concentration, and changes in enzyme activity are different readouts; an amplification claim should name its input, output and observation interval. [ref]
https://doi.org/10.1016/S0021-9258(19)77422-5. Rall and Sutherland (1958), methods: production and assay of cAMP
Articles by others on the same topic
There are currently no matching articles.