
A second messenger is a small intracellular molecule or ion that relays a received signal to target proteins. Its production, release, removal or binding changes its availability after signal reception. For a cell-surface receptor, distinguish the extracellular ligand, often called the first messenger, from the intracellular second messenger. An activated relay protein is not thereby a second messenger: the term identifies small chemical mediators, rather than every downstream component of signal transduction. [ref]
https://pubmed.ncbi.nlm.nih.gov/27481708/. Newton, Bootman and Scott, Second Messengers (2016): definition and classes
Two examples clarify what changes. A biological cell can make cAMP from ATP; alternatively, release of stored calcium ions can raise the free calcium concentration in its cytoplasm. The latter need not increase the total calcium content of the biological cell. Availability to target proteins, not merely the total amount present, carries the message. Removal and sequestration help terminate such signals. [ref]
https://www.ncbi.nlm.nih.gov/books/NBK10794/. Purves et al., Neuroscience, 2nd edition: second messengers and calcium storage
[ref]The experimental motivation is unusually tangible: can a hormone's effect be transferred to machinery that barely responds to the hormone itself? In Rall, Sutherland and Berthet's 1957 experiment, washed cat-liver particles were incubated with ATP and magnesium ions, with or without epinephrine and glucagon, two hormones. After five minutes at , the mixtures were heated in boiling water for three minutes, chilled, and separated to remove insoluble material. Small samples of the clarified extracts were transferred to a separate soluble dog-liver preparation, again supplied with ATP and magnesium ions. The readout was the change in glycogen phosphorylase activity over five minutes, not the amount of newly synthesized protein. [ref]
https://doi.org/10.1016/S0021-9258(18)65045-8. Rall, Sutherland and Berthet (1957), Figure 4 and pp. 470–471: preparation and transfer
The hormone-conditioned extract caused a larger increase in glycogen phosphorylase activity. Water, extract made without hormones, and hormones added directly to the soluble preparation produced smaller effects. These comparisons distinguish transferred activity from baseline activity, preparation effects and simple hormone carryover. [ref]
https://doi.org/10.1016/S0021-9258(18)65045-8. Rall, Sutherland and Berthet (1957), Figure 4: controls and observations
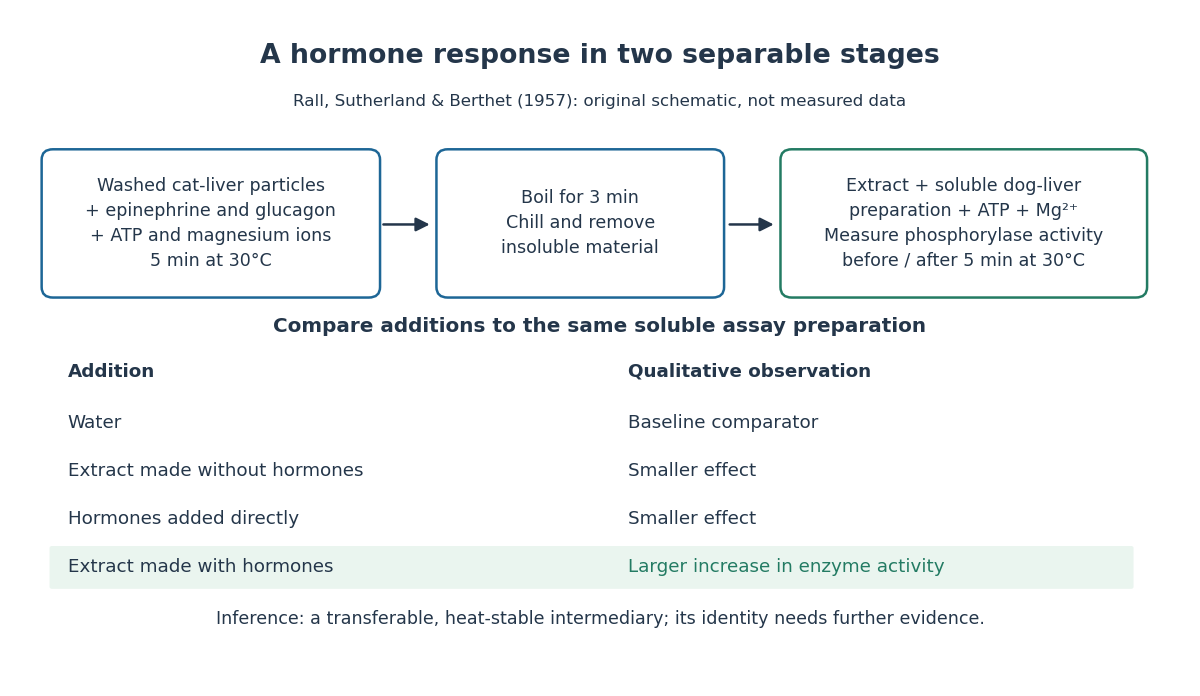

The inference is a transferable, heat-stable intermediary between the hormone-sensitive particles and the soluble machinery. This does not identify the intermediary merely from heat resistance, establish its direct target, or show that every hormone uses the same mechanism. Rall and Sutherland's 1958 paper reports the factor's identification as cAMP in accompanying chemical work, and follows its production from ATP. It also reports an important limit: washed heart and skeletal-muscle particles produced detectable cAMP with epinephrine under their test conditions, whereas brain particles produced similar amounts with and without it. Tissue and preparation matter. [ref]
https://doi.org/10.1016/S0021-9258(19)77422-5. Rall and Sutherland (1958), introduction and Table IV: cAMP identity and tissue-dependent responses
The useful and beautiful separation is between recognition and execution: an extracellular ligand can control intracellular enzymes through a chemically different intermediary. Making many second messenger molecules can support signal amplification, while different target proteins give the same mediator different consequences. A second messenger identifies a mode of relaying information; its presence alone does not specify the size or direction of the response. [ref]
https://pubmed.ncbi.nlm.nih.gov/27481708/. Newton, Bootman and Scott (2016): second messengers and their targets
New to topics? Read the docs here!