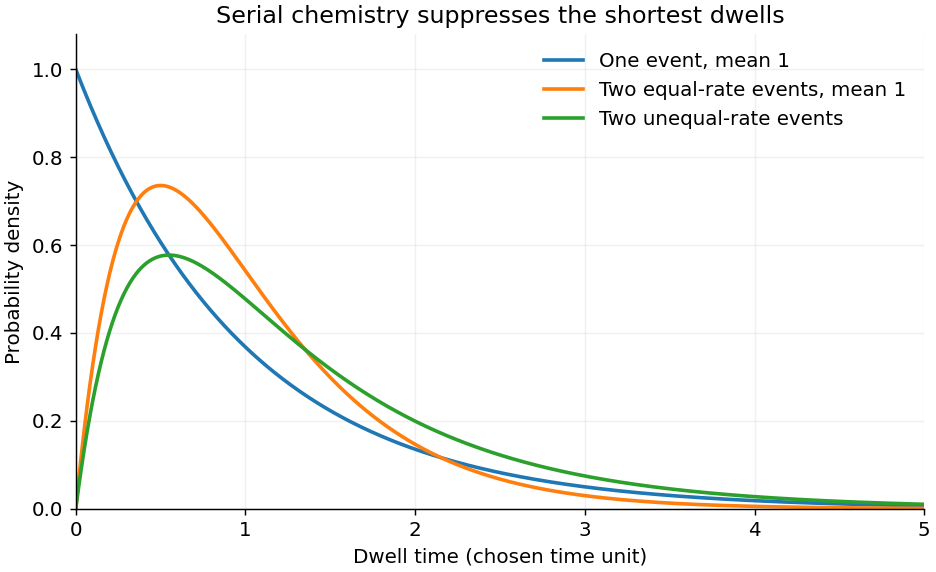
At saturating ATP, binding need no longer dominate the observed dwell, but saturation alone does not determine a dwell-time distribution. The standard interpretation of a distribution that rises from zero is that at least two sequential events remain rate limiting. Model a dwell as , where the independent waiting times are distributed according to exponential distributions with rates . Their convolution isThis hypoexponential distribution starts at zero, rises to a mode , then has an exponential tail. When the rates are equal, the continuous limit is the two-stage Erlang distribution,A single slow memoryless event instead gives , maximal at zero. Three 120-degree steps per revolution specify rotational stoichiometry, not three slow reactions within every dwell. The two-event interpretation is supported by the resolved catalytic-dwell chemical kinetics in the primary F1 experiment.[ref]
Resolution of distinct rotational substeps by submillisecond kinetic analysis of F1-ATPase by Ryohei Yasuda and others. 2001, abstract and Figure 8: two reactions occupy the catalytic dwell
The fit assumes sequential approximately irreversible events, constant rates during each dwell, negligible ATP-binding delay, negligible mechanical transit time, and detection of all relevant steps. Parallel pathways, backward transitions, inhibited states, probe drag and missed short dwells can change the histogram. The mathematical fit alone does not identify each event chemically or prove that two ATP molecules are hydrolyzed per step.

Articles by others on the same topic
There are currently no matching articles.