Define side as the higher proton electrochemical potential reservoir and side as the synthesis-side reservoir. For transfer at common temperature , define the positive downhill proton-motive force magnitude byHere is thermodynamic activity, is electric potential, is the molar gas constant and is the Faraday constant. Thus both a higher proton thermodynamic activity and a more positive electric potential on side contribute to the driving magnitude. This definition fixes the sign; conventions for a signed proton-motive force differ. The calculation under chemiosmosis separates these two contributions numerically.
Assume fixed reservoirs, tight mechanical energy coupling, one transported proton per subunit per revolution, and three ATP produced per revolution. Neglect leaks, slipping and membrane transport of the chemical reagents. Let be the local molar Gibbs free energy cost of ATP formation at the stipulated composition, pH and magnesium-binding convention. It is not necessarily the standard state value. Adding changes in the state function gives, per mole of complete turns,For this model net synthesis is thermodynamically favoured when . Equality is a reversible balance, not a promise of a useful reaction rate. A negative value establishes an available driving margin; it does not specify how fast the enzyme runs.
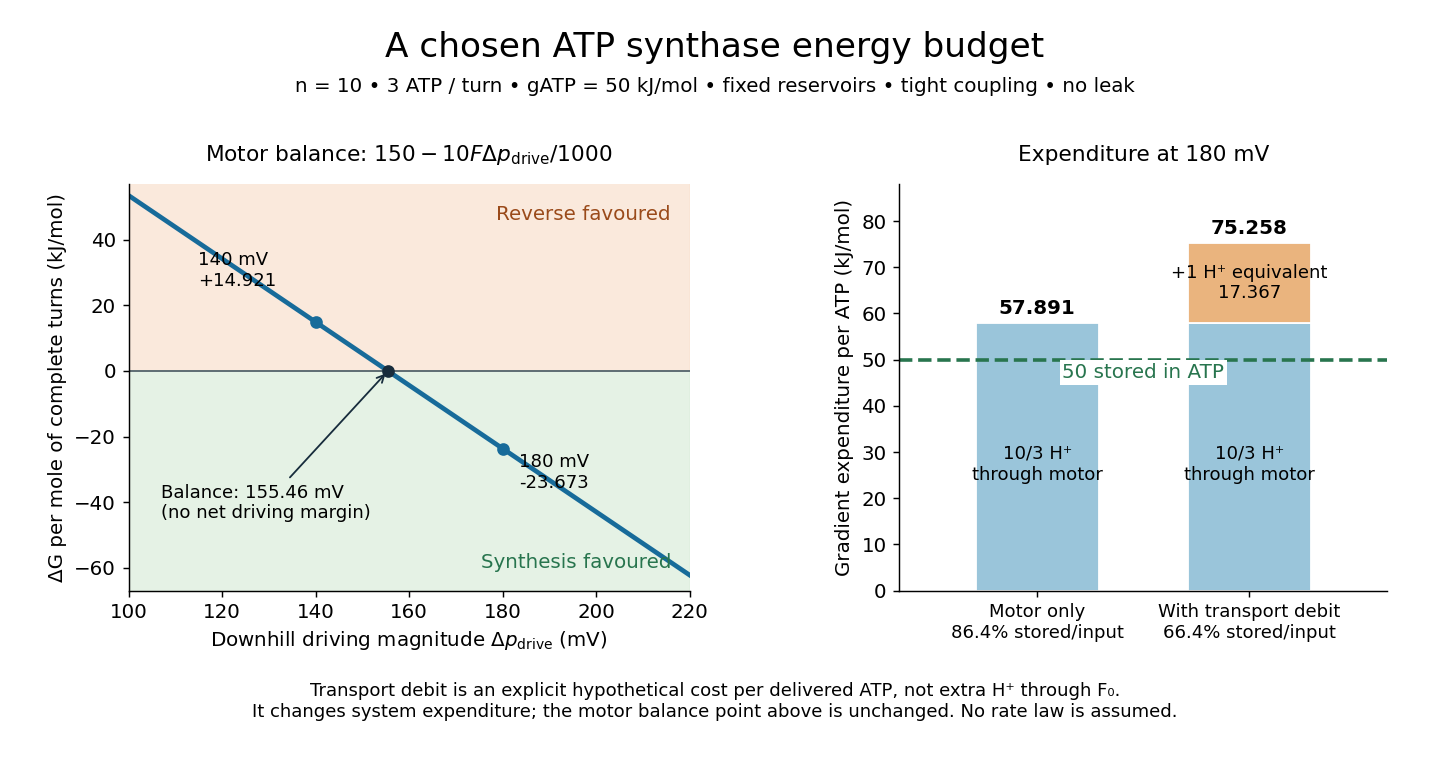
Choose , , and . These are illustrative inputs, not measurements of the preparation in the experiment below. Thenand . Per ATP, the ideal input is , leaving a driving margin of . The balance point isAt the same synthesis cycle instead has : the chosen reservoirs favour its reverse.

The machine is reversible: sufficient ATP hydrolysis can drive opposite rotation and pump protons uphill. Actual direction also depends on inhibition and available substrates; a weak proton-motive force need not make every intact enzyme immediately run backward. Respiratory uncoupling supplies a different failure mode: a parallel proton leak dissipates the gradient without productive shaft rotation.[ref]
Rotary catalysis of FoF1-ATP synthase by Rikiya Watanabe. Watanabe, 2013, p. 51 and Figure 2: reversal of the coupled motors
The motor budget is not the whole cost of ATP delivered outside a mitochondrion. Import of ADP and inorganic phosphate, and export of ATP, also draw on the electrochemical gradient.[ref]
The Mechanism of Oxidative Phosphorylation. Cooper, The Cell: A Molecular Approach, 2nd edition, Transport of Metabolites across the Inner Membrane, Figure 10.12
For a deliberately simplified system budget, assign these transports together one additional downhill-proton equivalent per delivered ATP, valued at the same . This is a chosen accounting convention, not a claim of one extra literal proton through , nor a universal transport stoichiometry. The total becomes equivalents and of gradient expenditure per delivered ATP at . The ratio of stored chemical free energy to that expenditure is , compared with for the motor alone. This system budget changes the resource expenditure, not the motor's balance point . Real transport terms require their own electrochemical potentials, and leaks add further cost. Articles by others on the same topic
There are currently no matching articles.