The per-capita net growth rate is . Thus is the low-density per-capita birth or recruitment rate, is the constant per-capita death or removal rate, and controls density-dependent suppression of recruitment. Both and have units of inverse time; has units of inverse population squared. The population scale halves the recruitment rate from its low-density value. Larger makes suppression important at smaller population sizes. These are interpretations of this phenomenological population dynamics model, rather than independently specified biological mechanisms.
Write . A steady state is a nonnegative zero of . If , the bracket is strictly negative for every , so only exists. If , there are exactly two nonnegative steady states,For an autonomous scalar ordinary differential equation, a steady state with is locally asymptotically stable, while one with is unstable. HereAt the positive steady state, use to obtainTherefore zero is stable for and unstable for , whereas the positive steady state is stable whenever it exists. At the omitted equality , ; zero is nonhyperbolic but still attracts every nonnegative initial state.
Linearizing at the positive steady state gives , so a small displacement decays as . The recovery time of a stable equilibrium is thereforeAs with fixed, and . Thus the equilibrium population approaches extinction and recovers increasingly slowly after small perturbations. This is critical slowing down. Exactly at the threshold the leading equation is , which gives algebraic decay instead of exponential recovery.
For , the sign of is positive on and negative on . Its graph passes through , has positive initial slope , and eventually behaves like . The phase line therefore points toward from both sides.
The vector field is continuously differentiable, so solutions are unique. No positive solution crosses either equilibrium; one starting below increases and stays below it, and one starting above it decreases and stays above it. These bounded solutions exist for all forward time and have a limit. By continuity of , any such limit must be a zero of : otherwise the derivative would stay bounded away from zero near the limit. The increasing solution is bounded below by its strictly positive initial value, excluding zero; the decreasing one stays above . ConsequentlyThe solution starting exactly at is constant. The zero initial condition remains at zero, which is why positivity is stipulated.
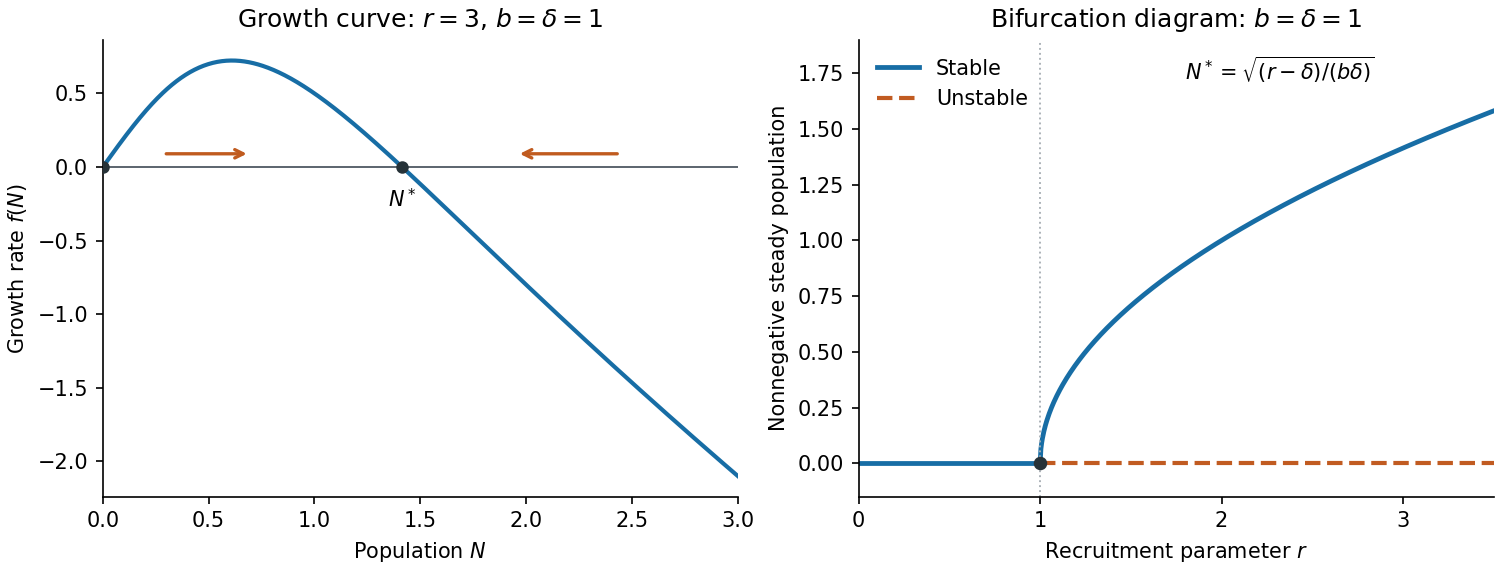

The nonnegative bifurcation diagram has the branch for every , stable for and unstable for . At the stable positive branch emerges:The figure in (iv) uses solid curves for stable steady states and a dashed curve for the unstable zero branch. At the meeting point the zero steady state is nonhyperbolic and attracts from the nonnegative side. If the equation is formally extended to negative , there is also the symmetric branch , giving a supercritical pitchfork bifurcation; its negative half is omitted in the biological diagram. This qualification avoids calling the single nonnegative square-root branch a full pitchfork by itself.
At a constant steady state , the discrete equation reduces toWrite . For , no nonzero real root is possible, so zero is the only real steady state. For the real roots areThus there is exactly one strictly positive steady state, . There are three real steady states in total, two of them nonnegative. At the only one is zero. This distinction keeps the positive-population statement separate from the count over all real numbers.
Let . At the positive steady state, , where . The two partial derivatives areThe first-order Taylor expansion with therefore givesEquivalently, the linearization on has matrix and characteristic polynomial .
For , . When , the roots of are real and lie strictly between zero and one. When , they are a complex-conjugate pair of modulus . Thus the positive steady state is linearly asymptotically stable exactly when , and unstable when . Since increases strictly with , the crossing occurs atAt the crossing,Every nonzero real linearized perturbation has period six. This establishes the intended linear stability threshold and linearized period six.
The nonlinear period-six claim in the printed paper does not follow, and is false as a local bifurcating-branch claim for this map. One can check this directly rather than infer a nonlinear period from the eigenvalues. At normalize , . The exact planar map isIts cubic Taylor expansion isHere is a concrete check of the sixfold return. Put , , andComposing the displayed cubic expansion six times cancels all quadratic terms and givesIn particularThe quartic coefficient is strictly negative. Hence, sufficiently near the equilibrium, every nonzero point has smaller after six iterations: the critical nonlinear map has no nearby nontrivial period-six orbit, and the equilibrium itself is locally attracting despite its neutral linearization.
One can also rule out a branch of small period-six orbits on either side of the crossing. Normalize about the positive equilibrium at each nearby , and put . The derivative of the sixth power of at is . Smooth dependence on therefore givesThe leading matrix has determinant . Both terms could vanish with only if , butThus its norm on nonzero is bounded below by a positive constant times , and the smaller remainder cannot cancel it. There is no nearby nonzero solution of . The eigenvalues satisfy the nonresonance conditions through order four, their moduli cross outward with increasing , and the cubic radial coefficient is negative. The standard Neimark–Sacker bifurcation theorem therefore gives a supercritical invariant closed curve. Its rotation is near the linear resonance ; it is not a local branch of exact period-six orbits.
Finally, the discrete population map does not preserve nonnegativity for arbitrary large lagged populations: can be negative. The positive-equilibrium stability conclusions above are local and do not assume a global positivity property that the formula lacks.
Articles by others on the same topic
There are currently no matching articles.