Diffusion and mobility. For a dilute isolated sphere in a Newtonian fluid, Stokes's law gives the drag magnitude , where is the dynamic viscosity and is the hydrodynamic radius. The mechanical mobility is therefore ; the translational hydrodynamic mobility matrix is .
To relate mobility to diffusion, put the particles in a weak external potential energy . Their drift speed is . For number density , the sum of drift and Fick's first law fluxes isAt thermal equilibrium, the Boltzmann distribution gives , and the net flux is zero. Substituting into yields . Thus the Stokes–Einstein relation isHere is the Boltzmann constant and is absolute temperature. The assumptions include a no-slip approximately spherical particle, a continuum fluid, a small particle Reynolds number, and negligible hydrodynamic interactions with other particles or boundaries.
Gravitational sedimentation. The buoyant force must be included, since the mass of displaced water is comparable to the protein mass. Using givesso the buoyant mass in the stated spherical model isThe drag coefficient is . At terminal speed, , soIgnoring buoyancy would give and would not use the supplied water density. This calculation treats the stated radius as both the hydrodynamic radius and the radius determining displaced volume; a real hydrated protein can require a separately measured partial specific volume.
Electrical drift. In the specified simple electrophoresis model, terminal force balance is . Thereforewhere is the electrophoretic mobility and the elementary electric charge. For the given positive beta-lactoglobulin charge,in the direction of the electric field. This exceeds the gravitational sedimentation speed by about .
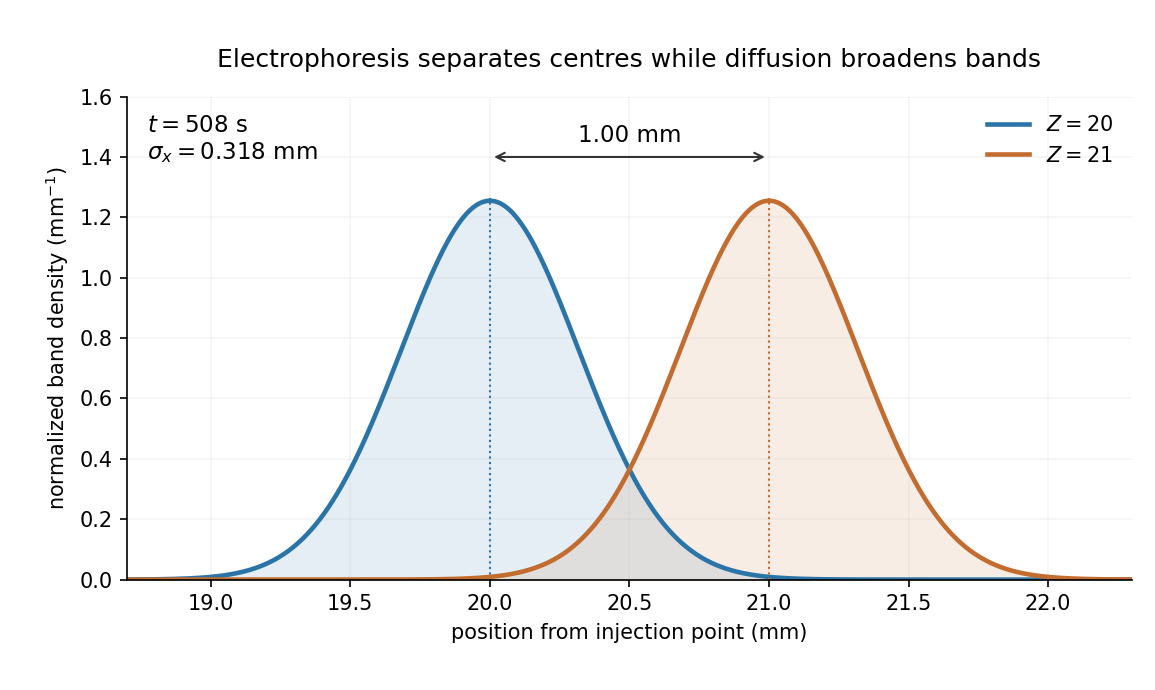
Separation time. The two populations have equal drag coefficients because their radii are equal. Their difference in drift speed is therefore set by one elementary charge:Starting with coincident band centres, their separation is . HenceAt that time the original band has travelled and the mutant . Their masses do not enter this ideal electrical force balance: equal-radius particles with different masses but the same charge would have equal electrophoretic mobility in this model.
Practical discrimination. A one-charge difference is enough for the stipulated separation, so the method is sensitive to mutations that change effective charge or friction. It cannot distinguish every mutation: substitutions that preserve charge and hydrodynamic size need not separate. Buffer pH changes protein ionization, and realistic electrophoresis also involves the ionic atmosphere, electro-osmosis, walls or gel interactions, and finite band widths.
For example, the Stokes–Einstein relation at gives . For an initially narrow band, diffusive broadening of electrophoretic bands givesat the calculated separation time. Thus the centres are about diffusion standard deviations apart, rather than forming infinitely sharp bands. The stated centre-separation criterion is achievable in the model, but actual resolution also depends on the loading width and other dispersion mechanisms.

Equivalent centrifugal acceleration. For the original protein to attain its electrical drift speed by sedimentation, its buoyant centrifugal force must equal :ConsequentlyThis is the acceleration at the protein's position in the rotating solution; no rotation rate can be assigned without a centrifuge radius. If the intended comparison is instead the relative separation speed of the two bands, use , since their displaced volumes are equal. Matching then gives . In that separation experiment the heavier original protein moves faster centrifugally, whereas the more highly charged mutant moves faster electrically.
Articles by others on the same topic
There are currently no matching articles.