An ecosystem is a system of interacting organisms and their nonliving surroundings. A pond study might include algae, fish, bacteria, water, dissolved chemical compounds and incoming light. The useful step is to state the boundary and time interval: the pond surface, bottom and shoreline might enclose the study region, but water, organisms and energy can cross them. The chosen boundary specifies what counts as internal storage, input or output; it does not make the ecosystem sealed. See Clark, Douglas and Choi, Biology 2e, 46.1: ecosystems and their components.
For a toy pond water budget over one day, begin with , add crossing inward, and remove crossing outward. With all other transfers omitted by assumption, the final amount is . The same bookkeeping asks whether a change inside an ecosystem came from internal processes or exchanges with its surroundings. Changing the boundary to include an upstream reservoir changes which transfers are internal, while preserving the accounting.
The difference between gross primary production and both autotrophic and heterotrophic respiration. A full storage budget must additionally account for disturbance and lateral transfers.
Carbon production remaining after subtracting autotrophic respiration from gross primary production. It need not remain stored, because consumers, decomposers and disturbance can return or export carbon.
The amount of carbon held in a specified pool or system. It is a stock, distinct from gross uptake or its rate of net change; large old stocks can coexist with small current fluxes.
Transfer of carbon into storage over a specified time horizon. Net sequestration requires uptake to exceed relevant losses under an explicit boundary; high photosynthesis alone does not establish it.
Maintenance or assessment of multiple ecosystem functions together. Functions can depend on different traits or conflict, so performance in one process cannot stand in for every other process.
A primary producer builds organic chemical compounds from inorganic sources. Photosynthetic algae, plants and cyanobacteria use light energy for this role through photosynthesis and carbon fixation. The role supplies new living material to a food web; it does not mean that the organism creates energy.
A consumer obtains organic material by feeding on other organisms or their products. A consumer feeding on primary producers is a primary consumer; one feeding on primary consumers is a secondary consumer. These names describe positions in a food chain, rather than permanent labels for a species.
A decomposer breaks down dead organic material and absorbs products of that breakdown; many bacteria and fungi perform this role. Decomposers connect detritus from different trophic levels to material recycling, so placing all decomposers at one final step of every food chain is misleading. See Clark, Douglas and Choi, Biology 2e, 46.1: grazing and detrital food webs.
An omnivore feeds on both primary producers and consumers. Its mixed diet explains why a trophic level need not be a whole number or a fixed label throughout an organism's life.
Detritus is nonliving organic material, including dead remains and organic wastes. It is a resource for decomposers, not itself an organism or a predator. In the illustrative food web, the dashed arrow from algae to detritus denotes a material transfer; the solid arrow from detritus to decomposers denotes resource use.
A trophic level describes feeding position relative to primary producers. Assign primary producers level 1; in the illustrated food chain, zooplankton occupy level 2, small fish level 3, and large fish level 4. Following a single feeding path adds one level at each step. The labels make dependence on the initial resource visible, but a branching food web can give an organism several feeding paths. See Clark, Douglas and Choi, Biology 2e, 46.1: feeding positions and branching food webs.
An omnivore can obtain food from more than one trophic level. As an explicitly assumed diet-weighted example, suppose an omnivore gets half its assimilated food energy from level-1 primary producers and half from level-2 consumers. Define its trophic level as one plus the weighted mean level of its food: . This computed position depends on the specified diet and weighting convention; it is not an immutable property of the species. A different life stage or diet can change it.
Energy flow tracks energy entering an ecosystem, passing through organisms and leaving its boundary. To see its quantitative effect, assume net production at one trophic level is and assume a transfer efficiency at each of two successive steps. Here measures the energy incorporated into new living material per unit area per day, after that level's own cellular respiration; it is not a count of organisms or a standing stock. The joule supplies the energy unit, with .
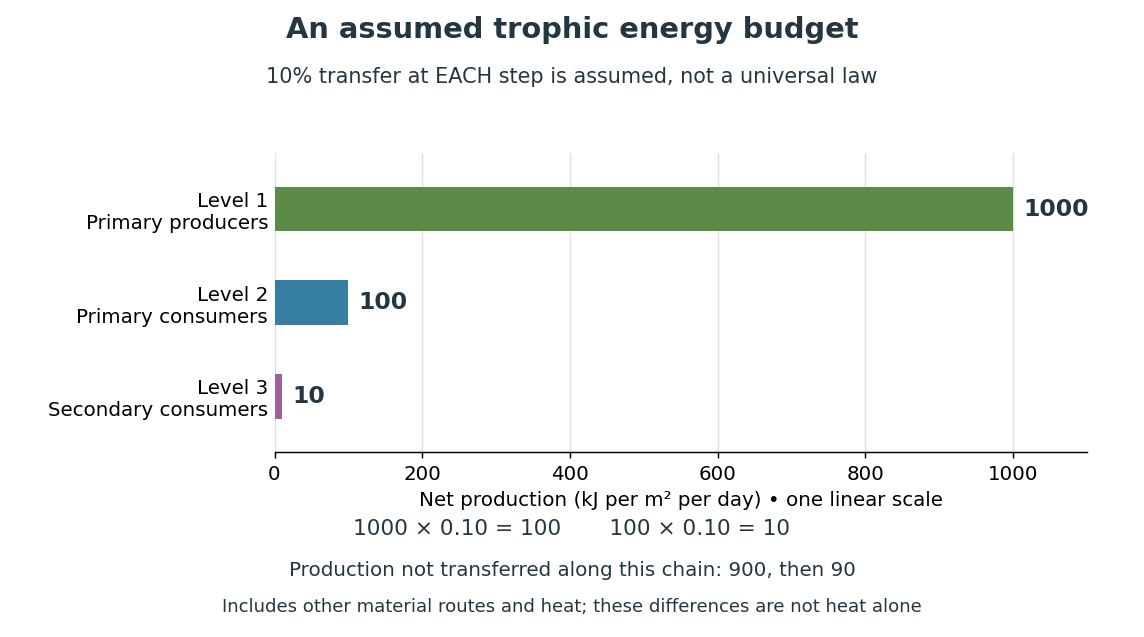

Only , or one percent, of the initial production reaches level 3 in this toy food chain. The first step leaves and the second outside the next level's new production. These differences can include uneaten material, wastes, and energy released as heat during cellular respiration; their separate amounts have not been assigned. Detritus can still carry energy to decomposers. The 10 percent efficiency is an assumption, not a universal law: transfer efficiencies vary with the organisms, food and conditions. The production ratio also differs from the fraction of an individual meal converted into growth. See Clark, Douglas and Choi, Biology 2e, 46.2: production and transfer efficiency.
The shrinking budget explains why supporting another trophic level requires enough production below it. It does not prove an exact maximum length for every food chain, particularly when a food web imports resources or has branching diets. Lindeman's 1942 paper grouped feeding relationships into trophic levels, compared transfers and cellular respiration, and emphasized the ecosystem as a unit connecting living and nonliving components. That viewpoint made different organisms comparable through a common energy budget. See Lindeman, The Trophic-Dynamic Aspect of Ecology (1942).
Material recycling and energy flow describe different bookkeeping. Carbon, nitrogen and phosphorus can be reused through chemical reactions and transfers between organisms and their surroundings. Energy transferred as heat is conserved, but is no longer the same store of chemical energy available to a consumer; photosynthetic primary producers need continuing light input. A decomposer helps recycle material and also releases heat through metabolism. Thus loss from one feeding budget means transfer into other forms or routes, never destruction of energy. See Clark, Douglas and Choi, Biology 2e, 46.3: material cycles. Conservation of energy applies to the whole accounting.
Zooplankton are drifting aquatic consumers, including small animals. In the illustrative food web, the chosen zooplankton feed on algae and serve as prey for small fish; this assumed diet is not a claim about every kind of zooplankton.
Phytoplankton are drifting aquatic organisms that carry out photosynthesis, including many algae. They can supply food to zooplankton in an ecosystem.
The standing stock of living phytoplankton, often expressed as carbon mass per water volume. Chlorophyll a is an accessible proxy, but its ratio to carbon is variable.
Articles by others on the same topic
There are currently no matching articles.