An organism is an individual living system, made of one biological cell or an integrated assembly of biological cells. An Escherichia coli cell is an entire organism; a neuron is normally a specialized part of an animal. Metabolism, regulated exchange through cell membranes, and inherited information connect these very different scales. See OpenStax Biology 2e, 1.2: living systems and levels of organization.
Keep two questions separate: how many biological cells make the organism, and how those biological cells are organized. A yeast and an Escherichia coli are both unicellular organisms, but the yeast is a eukaryote and the Escherichia coli a prokaryote. A plant and an animal are multicellular organisms with eukaryotic cellular organization. Neither distinction ranks organisms as better or worse: natural selection acts on reproduction in particular environments.
A historical grouping of predominantly unicellular eukaryotic organisms. Some include waterborne pathogens; the grouping is not a single modern evolutionary clade.
Organization of an organism as multiple associated cells, often with differentiated roles. Its evolution raises questions of reproductive alignment and control of within-body competition.
Passage through a single founding cell during a life cycle. It increases initial genetic similarity among descendants and restricts transmission of competing cell lineages, without preventing later mutation.
Differentiation between reproductive and nonreproductive cell lineages. Restricting which cells found descendants can reduce transmission of some within-body competitors.
A parasite with felids as definitive hosts; rodent odour-response experiments provide evidence relevant to, but not alone proof of, transmission-enhancing behavioural manipulation.
A unicellular organism is an organism whose living body consists of one biological cell. That biological cell maintains itself, grows and participates in reproduction; it is not merely one specialized component of a larger body. Escherichia coli and ordinary free-living Saccharomyces cerevisiae illustrate prokaryotic and eukaryotic examples respectively. Cellular organization and the number of biological cells are separate questions. See Clark, Douglas and Choi, Biology 2e, 4.1: cells as units of organisms.
How can one biological cell do enough to sustain an organism? Its cell membrane retains useful material while membrane transport allows exchange; metabolism transforms nutrients and supplies usable energy; gene expression makes proteins needed to maintain and rebuild the machinery. These functions operate together inside the same boundary. In Saccharomyces cerevisiae, for example, glucose can support alcoholic fermentation and production of ATP, while the cell cycle and budding produce descendants. A single biological cell therefore combines chemical processing, regulated exchange and inherited organization. See Alberts et al., Molecular Biology of the Cell (2002): universal cellular machinery and the experimental accounts under Saccharomyces cerevisiae and yeast.
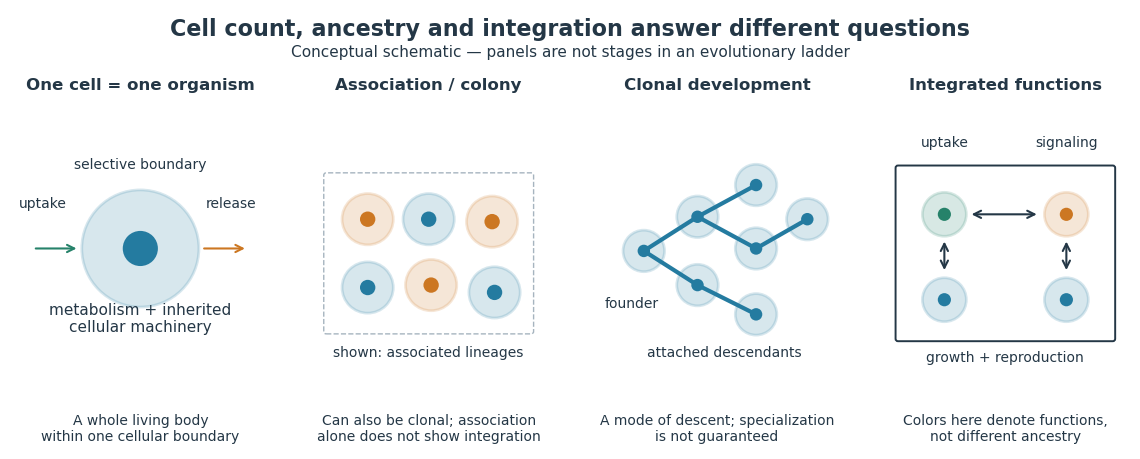
Being a unicellular organism does not mean isolated or independent of all other life. Unicellular organisms can interact and cooperate in groups. A biological colony describes association; clonal development describes descent; developmental integration describes coordination of the developing whole. Neither shared ancestry nor a visible clump alone establishes the latter. This distinction makes single-cell experiments easier to interpret: measuring the growth of one biological cell, the expansion of a group and the reproductive success of a reproducing cluster can answer different questions. See Queller and Strassmann, Beyond society: the evolution of organismality (2009): cooperation and the limits of simple organism criteria.
A multicellular organism has a body of multiple biological cells whose growth and activities are integrated into the life of the whole organism. Extensive cell differentiation is common in complex examples, but specialized biological cells are not a prerequisite for every simple form. Ask how the body develops, how its parts cooperate and how it produces descendants, rather than counting attached biological cells alone. The boundary with a biological colony depends on the degree of integration and the criteria being investigated; there is no universal cell-count threshold. See the Queller and Strassmann account cited under unicellular organism.
Specialization makes the whole capable of combinations that one general-purpose biological cell cannot achieve in the same way. In an animal, a neuron transmits signals while a red blood cell carries oxygen; each still requires a working cell membrane and metabolism. A mature mammalian red blood cell lacks a cell nucleus and mitochondria, illustrating how a useful part need not retain the equipment of a self-reproducing organism. See Clark, Douglas and Choi, Biology 2e, 40.2: red blood cell specialization. Cell differentiation generally involves different gene expression, rather than a different inherited genome for each function. Biological development must coordinate growth, position, interactions and specialization: increasing the number of biological cells is only one component. See Alberts et al., Molecular Biology of the Cell, chapter 21 (2002): construction of multicellular bodies.
A motivating experiment: select for a property of groups. Ratcliff, Denison, Borrello and Travisano's 2012 study began with Saccharomyces cerevisiae growing as unicellular organisms. Daily transfer favored rapidly settling material. Their initial protocol allowed a culture to settle for , discarded the upper , and transferred the bottom into fresh medium. After seven days, they instead sampled and centrifuged it at times gravitational acceleration for , again transferring the bottom . Faster settling made it more likely that a lineage would seed tomorrow's culture; the procedure selected a physical outcome without specifying how it must arise. These protocol details are explicitly recounted in Gulli, Herron and Ratcliff, Evolution of altruistic cooperation among nascent multicellular organisms (2019): original settling protocol.
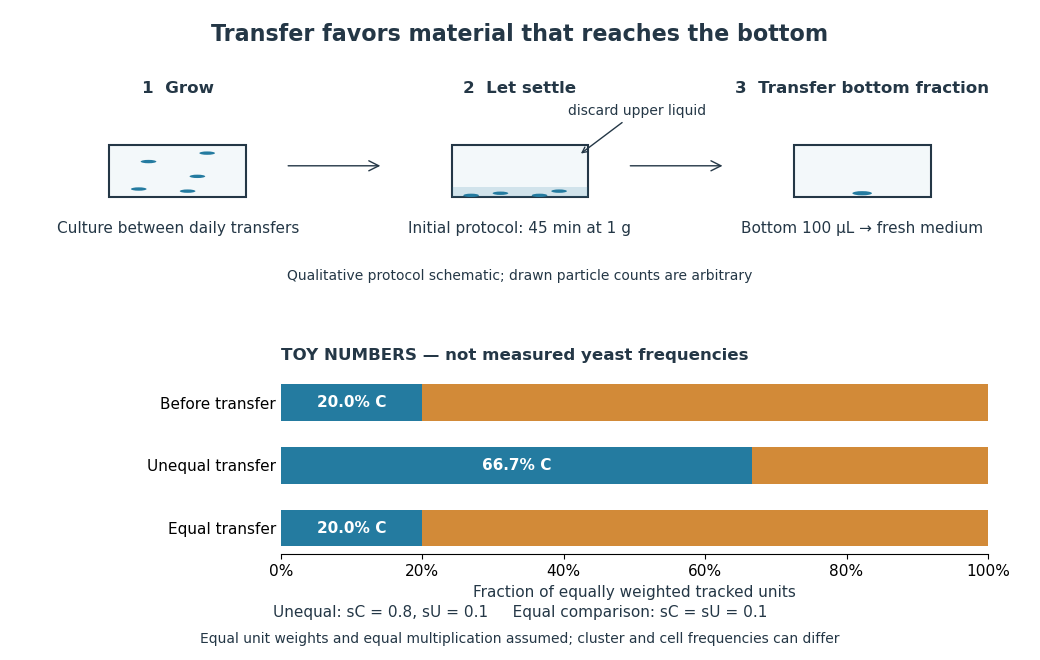
Settling selection and an explicitly stipulated enrichment example
. Original qualitative transfer schematic with toy numerical bars. The workflow represents the initial settling protocol described above. The lower panel assumes equally weighted tracked units and transfer probabilities and ; these values and the resulting frequencies are invented for explanation, not fitted to snowflake yeast measurements. The equal-transfer comparison is a model control, distinct from the experimental comparisons described below. Details.The primary 2012 paper reports snowflake yeast dominating all ten initial replicate populations by 60 transfers. To distinguish the joining of previously separate biological cells from clonal development, the researchers enzymatically separated clusters and followed individual biological cells for : attached descendants rebuilt clusters, with no such joining observed. Staining localized attachments at bud scars. Time-lapse observations also showed clusters releasing smaller multicellular offspring, called propagules; small clusters grew before they reproduced. See Ratcliff et al., Experimental evolution of multicellularity (2012), figures 1–3: emergence, development and reproduction.
The experimental comparisons ask different questions. Competition with the unicellular organism ancestor showed a reported advantage under settling selection. Without settling selection, the estimated disadvantage had a one-sided , so it was suggestive rather than decisive evidence of a cost. Separately, three populations derived from one evolved isolate retained the cluster form through 35 transfers without settling selection. That persistence tests stability, not whether clusters always outperform single biological cells. See Ratcliff et al. (2012), figure 2 and the cluster-formation results cited above.
A 2015 follow-up added a causal test: deleting the gene ACE2 in the unicellular organism ancestor produced snowflake yeast, while supplying functional ACE2 to one evolved isolate restored separation into single biological cells. Sequence changes altering the encoded protein were found in ACE2 in five of ten examined lineages; the study did not identify that same sequence-change mechanism in every lineage. The deletion and restoration comparisons support a mechanism beyond the observation that clusters settle quickly. See Ratcliff, Fankhauser, Rogers, Greig and Travisano, Origins of multicellular evolvability in snowflake yeast (2015), figure 1.
What follows, and what does not. The evidence supports inherited cluster formation, clonal development and a reproducing collective whose properties can respond to natural selection. Calling these simple multicellular organisms recognizes those demonstrated properties; it does not turn every clump into an animal or establish animal-like cell differentiation. This laboratory route also does not reconstruct the actual ancestry of animals or show that complex developmental integration must follow. The interesting achievement is narrower and testable: a change in how descendants remain connected creates a new scale at which growth and reproductive success can be measured.
For the toy figure, let be the fraction of tracked units of type C before transfer and let be the respective probabilities of transfer for C and U. Assume equally weighted units and equal multiplication between transfers. When overall transfer probability is nonzero, conditioning on transfer givesWith , and , the numerator is and the denominator , giving . If both types have the same nonzero transfer probability, the fraction stays . This is conditional probability, not a model of the full experimental life cycle: real cluster sizes, growth and fragmentation affect which quantity a frequency measures. In particular, a fraction of clusters is not automatically a fraction of biological cells.
Differentiation between cell lineages contributing to future organisms and those mainly maintaining the current body. Restricting transmission routes can help align cellular reproduction with organismal reproduction.
Clonal development builds a group through successive divisions of founding biological cells, rather than by gathering previously separate lineages. In snowflake yeast, daughter biological cells remain attached after budding. Common ancestry does not imply that every descendant remains genetically identical forever: new mutations can arise. See the 2015 study cited under multicellular organism.
Snowflake yeast are cluster-forming Saccharomyces cerevisiae with branching connections between mothers and attached daughter biological cells. They provide an experimental system for studying early transitions to simple multicellular organisms; see the protocol, observations and limits under multicellular organism.
Developmental integration here means coordination of cellular growth, organization and function into a developing whole. It describes what the parts do together, whereas clonal development describes how they descend from founders. Interactions through signal transduction can help coordinate cell differentiation; see the Alberts et al. development chapter cited under multicellular organism.
Cell differentiation is the acquisition of a specialized cell state, involving changes in structure, function and gene expression. A neuron and a red blood cell illustrate different outcomes: signaling and oxygen transport. Different functions usually do not require a different inherited DNA sequence for each function. The shared-genome principle concerns nucleated precursors and most nucleated descendants: a mature mammalian red blood cell has lost its cell nucleus and mitochondria, so it is not an example of two mature biological cells both retaining the same nuclear DNA. [ref]
Biology 2e by Mary Ann Clark and others. Biology 2e, §40.2, Red Blood Cells: specialization and absence of a nucleus and mitochondria at mammalian maturity
The puzzle is how a shared set of genes supports different jobs. Gene expression changes which RNA and proteins a biological cell produces, and in what amounts. A transcription factor can regulate several genes; different combinations of regulators can interpret the same signal differently. Stable regulatory patterns can persist through the cell cycle, providing memory of developmental history. Specialization therefore usually changes use of inherited information, rather than replacing the genome wholesale. [ref]
Molecular Biology of the Cell, 4th edition by Bruce Alberts and others. Alberts et al., The Molecular Genetic Mechanisms That Create Specialized Cell Types, subsections The Expression of a Set of Genes Can Be Coordinated by a Single Protein and Stable Patterns of Gene Expression Can Be Transmitted to Daughter Cells, and Summary
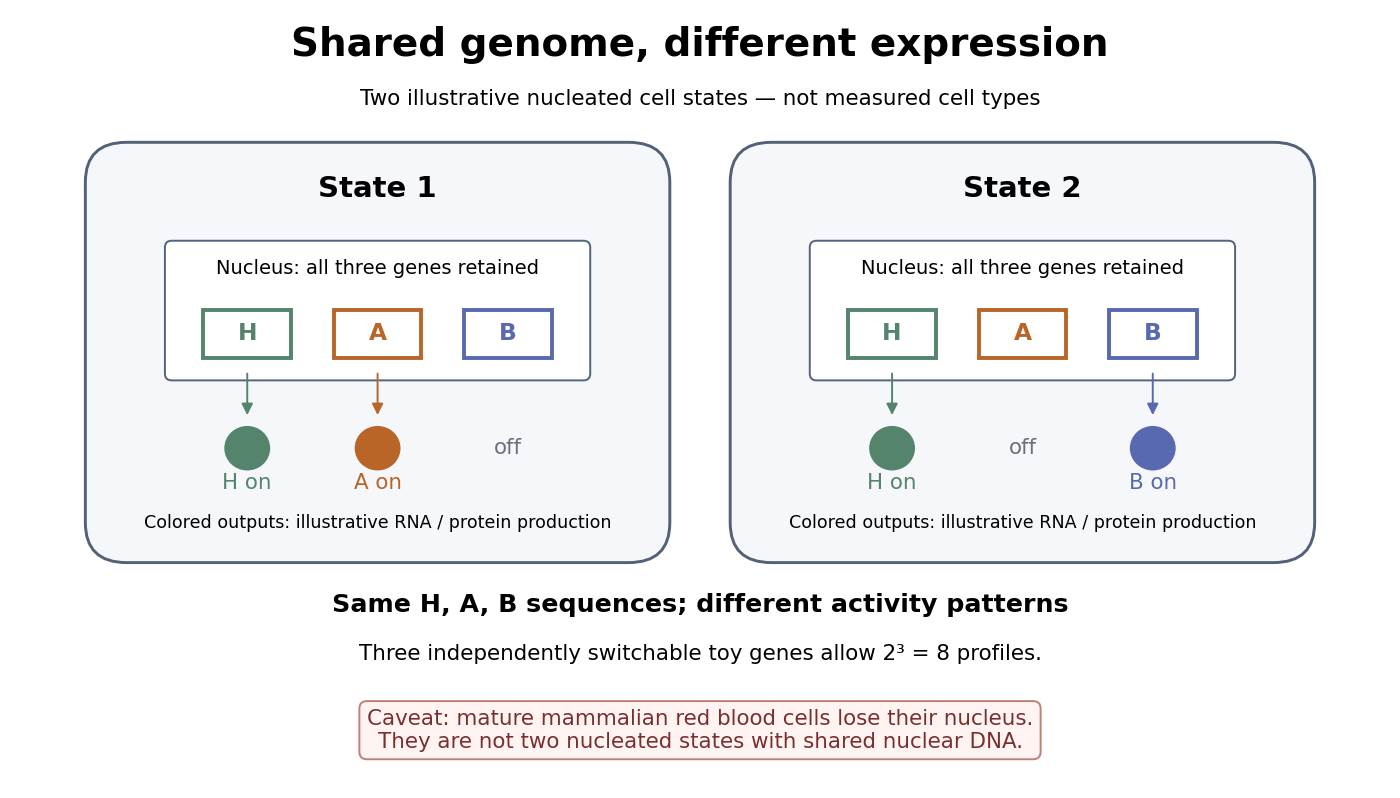
A small counting example separates sequence from activity. Suppose the same three toy genes are present in every nucleated biological cell, and independently assign each gene an on/off state. There are possible expression profiles with no DNA replacement. The figure shows only two: H and A on versus H and B on. Real gene expression is graded and coordinated, so this count illustrates possible descriptions, not a prediction of eight actual cell types. The interesting consequence is that a stable cell state can depend on how a shared record is used.
Stem cells combine self-renewal with production of differentiated descendants; progenitor cells generally have more restricted developmental options and renewal capacity. Neither term means that a biological cell must give rise to every cell type. Terminal differentiation denotes advanced specialization within a lineage, often accompanied by exit from the cell cycle. Cell fate concerns the developmental outcome of a biological cell or its descendants, whereas cell state describes its current properties. A temporary change in gene expression after signal transduction is not, by itself, proof of a new cell fate. [ref]
Anatomy and Physiology 2e by J. Gordon Betts and others. Anatomy and Physiology 2e, §3.6, Stem Cells and Differentiation: renewal, restricted differentiation potential and regulation of gene expression
A transition toward epithelial organisation and behaviour, potentially contributing to metastatic colonisation in particular cancer models.
The ability of cells to move among epithelial, mesenchymal and intermediate regulatory states. The benefit of a state can vary between dissemination, persistence and metastatic outgrowth.
A transition from an epithelial organisation toward more individually migratory cellular behaviour, involving changes in adhesion and polarity.
The developmental interval during which a cell can make a specified response to a signal. Absence of response outside the interval need not mean that the signal is absent.
Specification that depends on a cell's interactions with its surroundings. Neighbour exchange and controlled signal perturbation can test it causally.
Specification driven by information inherited within a cell, such as asymmetrically partitioned maternal material. It can coexist with external inputs later in development.
Cell fate is the developmental outcome of a biological cell or its descendants in a specified setting. What it normally becomes and what it can become after an experimental intervention are different questions. The intestinal nucleus transfer experiment tests potential after cellular reprogramming, rather than directly tracing the normal cell fate of the donor.
Persistence of a developmental choice. cell specification tests behaviour in a neutral environment; cell determination tests persistence in a viable conflicting environment.
Context-dependent capacity to change differentiated identity or developmental potential. Demonstrating a transition requires distinguishing conversion of a defined starting cell from selection of a rare pre-existing population.
Changes in intestinal epithelial potential that allow previously committed cells to restore a renewing stem-cell compartment under particular conditions.
Conversion between differentiated cellular identities. Whether a progenitor-like intermediate is traversed is an experimental question rather than part of a universal mechanism.
A return from a more committed state toward a less committed or progenitor-like state. Re-expression of one marker is weaker evidence than sustained renewal and functional lineage output.
A commitment demonstrated by retaining a fate in a conflicting environment that is viable and supplies the alternative developmental cues.
A provisional developmental commitment demonstrated operationally by adopting a fate in an appropriate neutral environment. It is weaker than cell determination.
A description of the normal developmental descendants of identified embryonic regions or cells. It reports realised fate, not the entire potential revealed by experimental transplantation.
Terminal differentiation is advanced specialization at the end of a developmental lineage. It often includes withdrawal from the cell cycle; the term does not mean that every nuclear gene needed for another cell fate has been deleted. A mature mammalian red blood cell is an especially restrictive example because it lacks a cell nucleus; the intestinal nucleus transfer experiment used nucleated donors.
Cellular reprogramming changes an established cell state so that a different developmental program becomes accessible. Experimentally induced cellular reprogramming must be distinguished from the ordinary progression of cell differentiation. An ovum's cytoplasm can reset aspects of a transferred cell nucleus; this does not mean that a specialized donor normally returns to an early developmental state in its original surroundings. [ref]
Mature cells can be reprogrammed to become pluripotent by Nobel Assembly at Karolinska Institutet. Nobel Assembly, Mature cells can be reprogrammed to become pluripotent, Scientific background: Gurdon nuclear transfer and distinction between differentiation and reprogramming
Large-scale changes in chromatin-associated regulatory states and DNA methylation during a developmental transition. Loss of methylation is not by itself a measurement of reduced transcription.
Somatic cell nuclear transfer introduces a body-cell cell nucleus into an ovum whose own nuclear contribution has been removed or inactivated. The donor nuclear genome and recipient cytoplasm have different origins; successful development does not show that the donor cell nucleus acts independently of the recipient's machinery.
Can a specialized donor still supply information for other cell types? The 1962 The Developmental Capacity of Nuclei taken from Intestinal Epithelium Cells of Feeding Tadpoles by J. B. Gurdon used mid-intestinal cells of feeding Xenopus laevis tadpoles. Donors were recognized by columnar shape, basal cell nuclei and a striated absorptive border. Dissociation used Versene solution; this made individual donors accessible. The readout was subsequent development, including normal feeding tadpoles, rather than just division or survival. [ref]
The Developmental Capacity of Nuclei taken from Intestinal Epithelium Cells of Feeding Tadpoles by J. B. Gurdon. Gurdon (1962), Material and Methods and Normal tadpoles; inspected primary text reproduced in the indexed Paperity preview
Apparatus and intervention. A microscope with ultraviolet illumination directed light at the surface region containing the unfertilized ovum's chromosomes, inactivating the recipient nuclear contribution. Irradiation also softened the surrounding jelly so a glass micropipette could enter. The pipette delivered donor nuclear material into recipient cytoplasm. In the technique's validation, fertilizing irradiated eggs produced haploid embryos, supporting destruction of the maternal nuclear contribution. This is inactivation, not a diagram of surgically removing an intact cell nucleus. [ref]
The Egg and the Nucleus: A Battle for Supremacy by J. B. Gurdon. Gurdon, The Egg and the Nucleus: A Battle for Supremacy, The Technique of Nuclear Transfer in Xenopus; indexed authored Nobel lecture text inspected
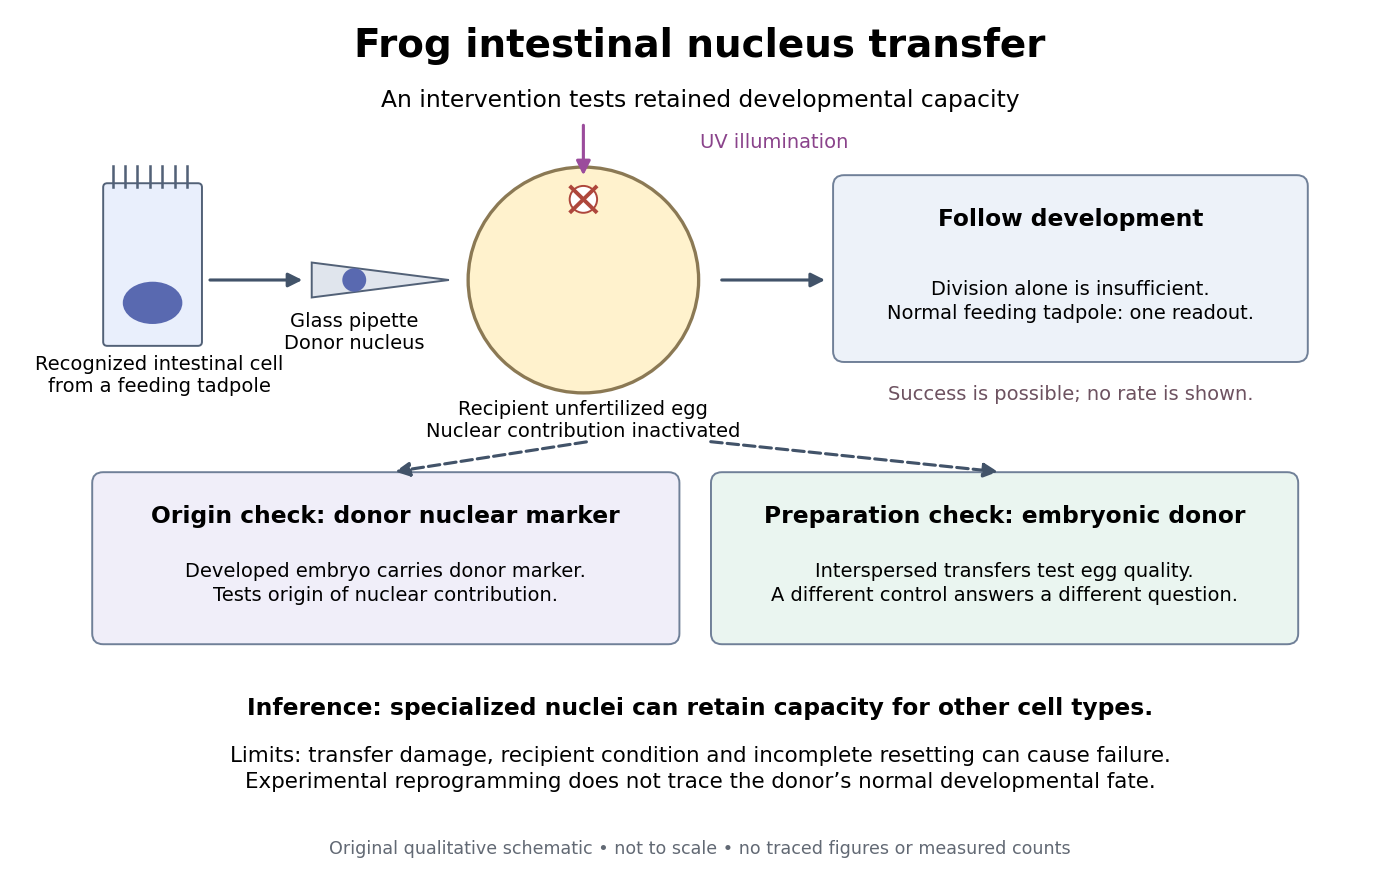
Somatic cell nuclear transfer: intervention, developmental readout and distinct controls
. Original apparatus-and-inference schematic, not a tracing of an experimental photograph. The ultraviolet beam indicates inactivation of recipient nuclear material; the injection pipette supplies a donor cell nucleus. Donor nuclear markers test origin; interspersed embryonic-donor transfers test recipient quality. Successful development is a possible outcome, not an asserted success rate. The figure omits exact dimensions, light dose and many technical steps. Details.Controls ask different questions. Donor cell nuclei carried a marker absent from recipients; post-blastula embryos carried that marker. The marker distinguished diploid donors with one nucleolus per cell nucleus from the usual two-nucleolus recipient background, rather than mistaking one nucleolus for proof of a haploid state. [ref]
The Egg and the Nucleus: A Battle for Supremacy by J. B. Gurdon. Gurdon, Nobel lecture, The Technique of Nuclear Transfer in Xenopus, p. 233: one-nucleolus diploid marker and its use to establish donor nuclear origin
Interspersed transfers of blastula or later embryonic cell nuclei checked variable recipient quality. A positive embryonic-donor control thus tests the preparation, while the marker tests donor origin. Abnormal development remained common. Neither control establishes universal transfer competence. [ref]The Developmental Capacity of Nuclei taken from Intestinal Epithelium Cells of Feeding Tadpoles by J. B. Gurdon. Gurdon (1962), Material and Methods (nuclear marker), Results (interspersed embryonic controls), and Normal tadpoles (abnormal outcomes); primary text inspected through the indexed preview
Inference and limits. A successful marked donor demonstrates that specialization had not irreversibly removed all information required to build other cell types. Failure is less decisive: transfer damage, recipient condition and incomplete cellular reprogramming can also prevent development. The marker identifies nuclear origin; it is not a complete DNA sequence comparison. The experiment tests donor nuclear potential in an altered cytoplasm, rather than normal donor cell fate, a universal capacity of every donor, or development from a mature mammalian red blood cell. The Nobel account also describes serial transfers through embryonic intermediates; these must not be silently combined with direct transfers into one success rate. [ref]
Mature cells can be reprogrammed to become pluripotent by Nobel Assembly at Karolinska Institutet. Nobel Assembly, Scientific background, Gurdon's nuclear-transfer experiments and serial transplantation
A biological colony is an associated group of organisms or biological cells. The name alone specifies neither cell differentiation nor a particular mode of biological development. A colony can arise from related descendants or from previously separate members; see clonal development and the Queller and Strassmann discussion cited under unicellular organism.
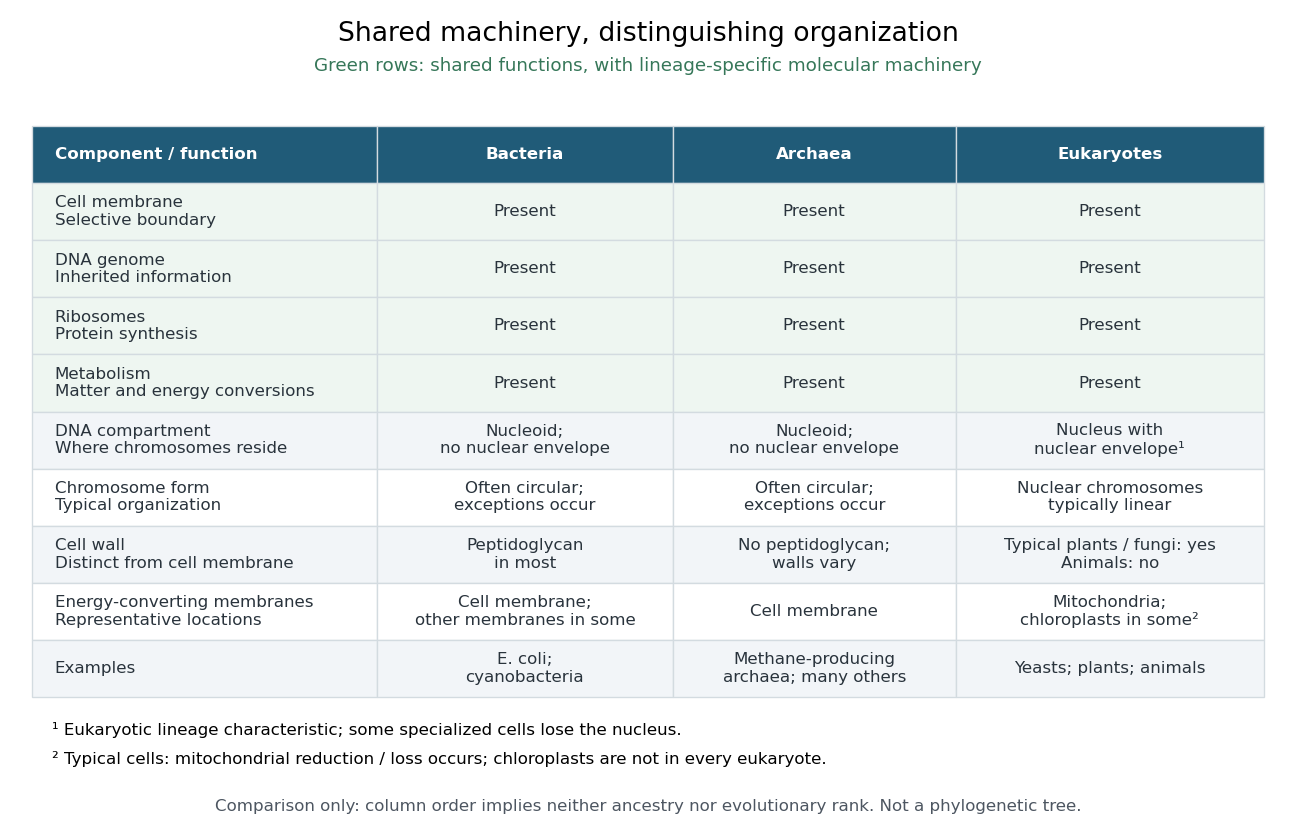
A prokaryote is an organism whose biological cells lack a membrane-bounded cell nucleus. The DNA of its chromosomes occupies a nucleoid within the cytoplasm. Bacteria and archaea have this cellular organization. Both contain ribosomes that perform biological translation and a selective cell membrane; neither is a bag of unorganized chemicals. See OpenStax Biology 2e, 4.2: prokaryotic organization.
The word prokaryotic describes organization, not a single exclusive clade. Grouping bacteria and archaea by the absence of a cell nucleus is useful for comparing biological cells, but does not establish that they share a more recent ancestor with one another than either does with eukaryotes. See three-domain system and two-domain system for the different ancestry models.
Prokaryotic does not mean membrane-free. Cyanobacteria contain internal thylakoid membranes for oxygenic photosynthesis, despite lacking chloroplasts and a cell nucleus. Many prokaryotes have circular chromosomes, but circular shape and a single chromosome are not defining requirements. See OpenStax Biology 2e, 22.2: bacterial and archaeal structures.
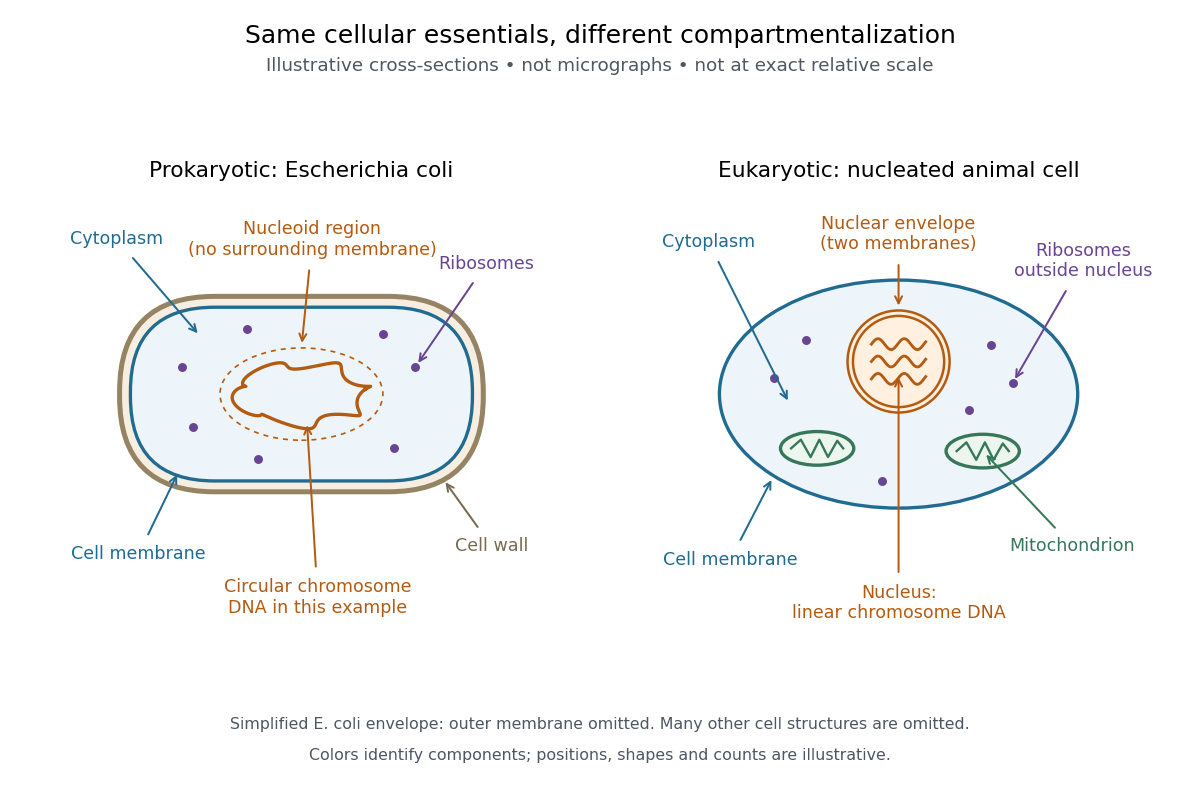
Bacteria are a major evolutionary lineage of organisms with prokaryotic cellular organization. Escherichia coli and cyanobacteria illustrate its variety: the same broad cellular plan supports different kinds of metabolism. Most bacteria have a cell wall containing peptidoglycan; archaea do not have peptidoglycan walls. A cell wall and a cell membrane are distinct structures, and some bacteria lack a cell wall. See OpenStax Biology 2e, 22.2: bacterial envelopes.
The usefulness of recognizing bacteria extends beyond naming: it identifies a shared evolutionary background for comparing genes, proteins and cellular mechanisms. A familiar shape or the absence of a cell nucleus alone cannot distinguish bacteria from archaea; molecular comparisons, including ribosomal RNA, supply additional evidence.
A group of bacteria capable of oxidative production of acetic acid from ethanol; particular cultures can contain several species.
A historical designation used for the vinegar-forming surface growth. It should not be assumed to identify every modern vinegar organism as one species.
Historical grouping of minute moving elongated or sinuous organisms; not coextensive with the modern genus Vibrio.
The bacterial species associated with tuberculosis. Bulk lesion chemistry does not by itself establish its presence.
The bacterial cause of typhoid fever.
A bacterial species that is a natural host of Bacillus virus phi29. The host identity matters when distinguishing that bacteriophage from unrelated Escherichia coli bacteriophages.
A functional grouping of bacteria able to establish nitrogen-fixing root-nodule symbioses with compatible legumes. Compatibility and fixation effectiveness vary between partners.
A bacterial species used as a model of respiratory extracellular electron transfer, including the MtrCAB pathway.
A microbial community associated with a self-produced extracellular matrix. Local exposure, growth state and population heterogeneity can change responses to antimicrobial treatment.
The bacterium responsible for American foulbrood.
Coxiella burnetii is a specialized intracellular bacterium whose replication was achieved in host-cell-free medium. Its natural intracellular niche must therefore be distinguished from an absolute biochemical requirement for a living host in all culture conditions.
Buchnera aphidicola is an intracellular aphid symbiont associated with nutritional complementation. Its reduced genome retains functions relevant to amino-acid provision, illustrating a host-dependent mutualism rather than simply a pathogenic strategy.
Rickettsia parkeri is a spotted-fever-group intracellular bacterium used to study Sca2-dependent actin assembly. Its motility machinery should not be generalized to every rickettsial species.
Chlamydia is a bacterial genus containing intracellular species with developmental transitions between infectious and replicative forms.
Rickettsia prowazekii is an intracellular bacterium with extensive biosynthetic losses but retained respiratory and citric-acid-cycle functions. Its cytosolic niche and metabolic inventory differ from those of inclusion-resident Chlamydia.
Chlamydia trachomatis is an intracellular bacterium that replicates within a modified host-cell inclusion and alternates between infectious and replicative forms.
Pseudomonas aeruginosa is a bacterium with flexible central carbon metabolism. Its isocitrate branchpoint includes two regulated dehydrogenase routes and a glyoxylate shunt.
Alphaproteobacteria are a bacterial group implicated in the ancestry of mitochondria. This relationship concerns common descent, not descent from a named modern member of Alphaproteobacteria.
Escherichia coli, often abbreviated E. coli, is a bacterial species widely used to study DNA replication and gene expression. Its chromosome is in a nucleoid, and its ribosomes work in the cytoplasm, outside any cell nucleus. A result from one laboratory strain should not automatically be generalized to every member of the species.
The original 1997 report by Blattner and colleagues presented the K-12 MG1655 genome sequence as a circular chromosome of base pairs. See Blattner laboratory: original K-12 sequence and 1997 paper. As a bookkeeping example, one complete round of DNA replication from one such chromosome produces two daughter sequence copies totaling base pairs. This is twice the copied material, not twice the length of the reference genome; it does not specify the instantaneous DNA content of a rapidly growing E. coli cell.
Cyanobacteria are bacteria that perform oxygenic photosynthesis: light-dependent reactions release oxygen from water. Their photosynthetic machinery operates on thylakoid membranes without a chloroplast or a cell nucleus. This is a particularly useful counterexample to equating photosynthesis with being a plant. Chloroplasts descend from an ancestral cyanobacterial partner through endosymbiosis; present-day cyanobacteria are independent descendants, rather than chloroplasts waiting to become plants. See Alberts et al., Molecular Biology of the Cell: chloroplasts and cyanobacteria.
A genus of oxygenic photosynthetic bacteria. The strain PCC 6803 is a common experimental system for photosynthesis and electron-export studies.
A marine cyanobacterial genus used in experiments on protection supplied by peroxide-removing microbes.
Typical Gram-positive bacteria have a relatively thick peptidoglycan layer outside the cell membrane, without the bacterial outer membrane of typical Gram-negative bacteria. This is a representative cell envelope pattern, not a complete description of every member of bacteria.
Typical Gram-negative bacteria have a relatively thin peptidoglycan layer between the cell membrane and a bacterial outer membrane.
Bacillus megaterium is the historical species name used for strain KM in the lysozyme wall-removal experiment.
Archaea are a major evolutionary lineage distinct from bacteria. The cellular comparison here concerns the prokaryotic members of archaea; see two-domain system for broader clade usage. Their biological cells have a nucleoid rather than a membrane-bounded cell nucleus, yet aspects of DNA replication, transcription and biological translation resemble those of eukaryotes. Their characteristic lipids differ chemically from the usual bacterial membrane lipids, and their cell walls, when present, lack peptidoglycan. See OpenStax Biology 2e, 22.2: archaeal distinctions.
Some archaea perform methanogenesis, producing methane as part of their metabolism. Archaea also inhabit ordinary soils and oceans: extreme habitats do not define the lineage. See OpenStax Biology 2e, 22.1: moderate and extreme environments. Woese and Fox's 1977 analysis of ribosomal RNA distinguished the methanogenic group they called archaebacteria from typical bacteria. Their proposed three primary lines of descent were a historical interpretation, rather than the final resolution of deep phylogenetics. See Woese and Fox, 1977: Phylogenetic structure of the prokaryotic domain.
Asgard archaea are an archaeal group important in studies of eukaryotic origins. Molecular comparisons connect their genes to the nuclear lineage of eukaryotes, rather than making modern Asgard archaea the direct ancestors of modern animals or plants. See the original analysis cited under two-domain system.
A eukaryote is an organism belonging to the lineage characterized by a membrane-bounded cell nucleus and extensive cellular compartmentalization. A nuclear envelope surrounds the nuclear genome; nuclear chromosomes are typically linear. Ribosomes perform biological translation outside the cell nucleus. See OpenStax Microbiology, 3.4: nuclear organization and protein synthesis. Specialized biological cells can lose their cell nucleus, as mature mammalian red blood cells do, while remaining parts of eukaryotic organisms; see OpenStax Biology 2e, 40.2: mature red blood cells.
Yeasts, plants and animals are all eukaryotes. Typical cells in these groups have mitochondria, but chloroplasts belong to photosynthetic plant and algae lineages, not to every eukaryote. A cell wall occurs in typical plant and fungus cells but is absent from animal cells. These are comparisons of representative cells, not a checklist every specialized cell must satisfy. See OpenStax Biology 2e, 4.3: nucleus, organelles and representative cells.
The interesting feature is controlled separation: cell membranes and organelle membranes let different cellular processes occupy distinct compartments while membrane transport connects them. The evolution of eukaryotes also involved partnership: mitochondria descend from a bacterial endosymbiosis. Modern phylogenetics supports an archaeal ancestry for the nuclear lineage, alongside this bacterial contribution; see two-domain system. Thus the history of a whole eukaryote cannot be read as the history of just one of its genes.
A member of the ciliate lineage, characterized in typical examples by cilia and distinct germline and somatic nuclear systems. Sexual and nuclear-development details differ across species.
The separation of germline and somatic nuclear functions in distinct nuclei. In ciliates, a micronucleus preserves germline inheritance while a macronucleus supports vegetative expression.
The somatic nuclear compartment of a ciliate, often highly polyploid. Development can involve DNA elimination and amplification, and vegetative inheritance can involve amitotic division.
The germline nuclear compartment of a ciliate. It contributes meiotic and zygotic inheritance, rather than supplying most vegetative transcription.
A ciliate genus used to study nuclear dimorphism, conjugation, autogamy and epigenetic inheritance. Nuclear-cycle details and mating-type mechanisms differ between species.
A model ciliate in which small-RNA-guided developmental DNA elimination contributes to mating-type inheritance, including regulation of the mtA promoter.
A model ciliate with seven mating types and developmentally programmed somatic genome rearrangement. Compatible cells exchange pronuclei during conjugation; population increase occurs separately through fission.
Camelina sativa is an oilseed plant used to investigate engineered accumulation of long-chain omega-3 fatty acids. Agronomic productivity and the percentage of a target in seed oil are distinct measurements.
A dinoflagellate belongs to a eukaryotic lineage notable for unusual nuclear chromosome organization. Many species have persistently condensed DNA with low bulk histone abundance, while retained histones and alternative nucleoproteins caution against a universal histone-free description.
A fungus is a eukaryote that obtains nutrients by absorption rather than photosynthesis. Fungi include unicellular yeasts and multicellular forms. Their cell walls differ from bacterial peptidoglycan walls; having a cell wall does not make a fungus a plant. See OpenStax Biology 2e, 24.1: fungal nutrition and organization.
A fungus adapted to infect keratinised tissues. Malassezia associated with pityriasis versicolor is not thereby a dermatophyte.
A genus of dermatophytes; it should not be inferred from the nineteenth-century name Microsporon furfur used for pityriasis versicolor.
Yeasts are fungi whose growth is predominantly unicellular, commonly through budding or division into two cells. The word describes a growth form across different fungal lineages, rather than one species or an exclusive clade; some fungi can switch between unicellular and filamentous growth. Thus Saccharomyces cerevisiae is a yeast, but yeast is not another name for that one species. See Kurtzman, Fell and Boekhout, The Yeasts, chapter 1 (2011): definition and classification.
A yeast cell has eukaryotic organization, including a cell nucleus, mitochondria and a cell wall. Small size and a unicellular lifestyle do not make it a member of bacteria. These compartments let an experimentally accessible biological cell retain much of the organization shared with other eukaryotes. See Clark, Douglas and Choi, Biology 2e, 24.1: fungal cells and yeast growth.
A motivating experiment: can fermentation continue without intact yeast cells? In 1897, Eduard Buchner ground brewers' yeast with quartz sand and diatomite, added water, and pressed out a liquid extract. Adding concentrated cane sugar produced carbon dioxide after 15–60 minutes. A cell-retaining filter still yielded an active filtrate: with sterilized cane sugar in an icebox, fermentation began after about a day. Saturated lactose gave no observed fermentation. These are reported observations, not invented control results. See Buchner, Alcoholic fermentation without yeast cells (1897), translated excerpt hosted by Carmen Giunta.
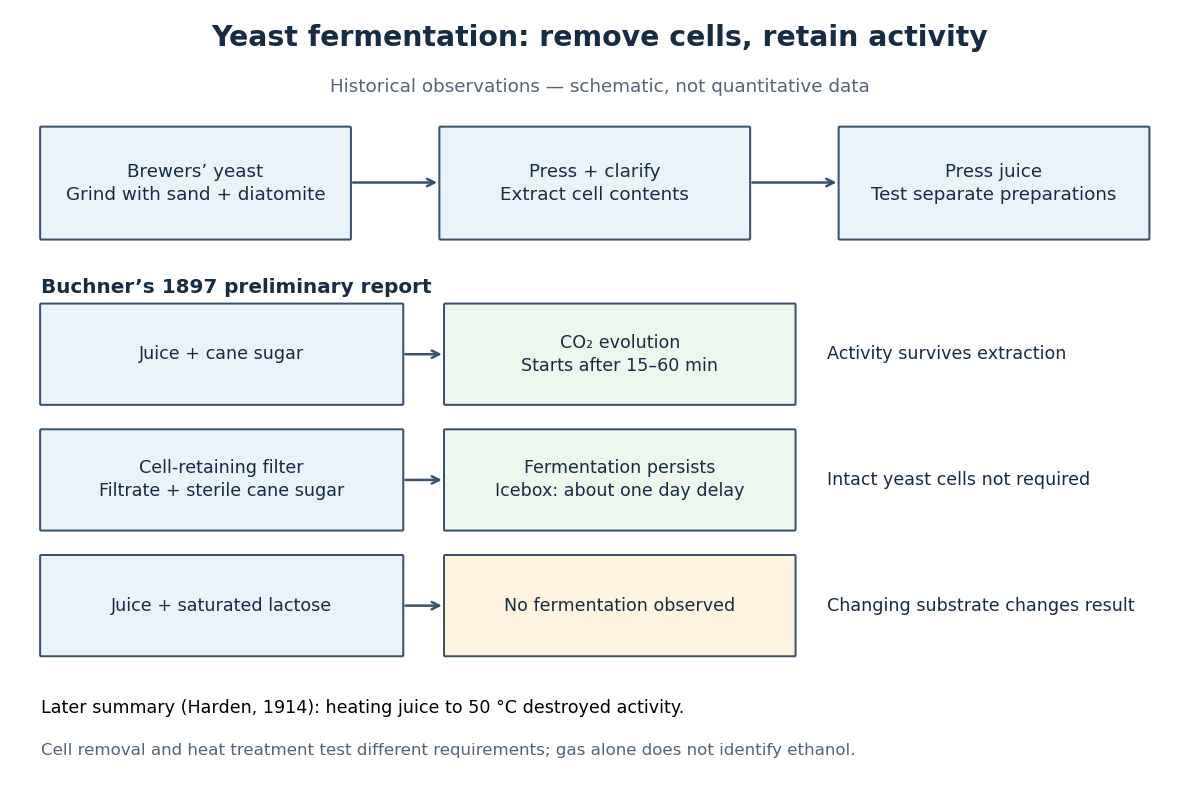
The filtration comparison addresses the objection that surviving intact yeast cells caused the activity. The lactose comparison tests substrate dependence; it is not a no-sugar blank, nor a comparison at matched sugar concentrations. A proposed modern follow-up would also compare the same extract with and without added sugar, accounting for material already in the extract. That is an experimental suggestion, not a result attributed to Buchner. His report specifies brewers' yeast; it does not identify the preparation here as a pure Saccharomyces cerevisiae strain.
Heat treatment asks a different question: does destroying activity in the extract stop fermentation? Buchner's preliminary report described weak or absent activity after heating and filtration, rather than one clean universal threshold. Harden's 1914 account of the subsequent work summarized loss of activity on heating the juice to . Harden also described requirements for both enzymes and coenzymes. Cell-free therefore means neither chemical-free nor a preparation containing one purified enzyme. See Arthur Harden, Alcoholic Fermentation (1914), chapters II and VI: cell-free activity and the fermenting complex.
The inference is that extracted cellular machinery can sustain these chemical reactions without an intact living biological cell. This does not show that the extract reproduces, grows or maintains itself like a yeast. Moreover, gas evolution alone does not identify ethanol: cellular respiration can also release carbon dioxide. Product identification is a separate measurement; Harden's account describes both ethanol and carbon dioxide as products of cell-free alcoholic fermentation. The beautiful separation is between the organism that produces and maintains the machinery and the machinery that catalyzes a particular transformation.
Yeasts that grow a daughter biological cell as a bud from a mother. Bud emergence, daughter-cell growth and successful completion of division are distinct endpoints.
Formation and growth of a daughter-cell bud. A visible bud is evidence of initial polarized cell growth but does not establish normal cytokinesis or long-term proliferative capacity.
Schizosaccharomyces pombe is a yeast species used as a model organism. It supplies the candidate genes in the yeast cross-species complementation experiment; the recipient remains Saccharomyces cerevisiae.
Saccharomyces cerevisiae is a particular species of yeast, used in baking, brewing and laboratory research. During ordinary vegetative growth it reproduces by budding: a smaller daughter grows from the mother before separation. Laboratory strains can be maintained as either haploid or diploid biological cells. This makes it possible to investigate genes in a single eukaryote, then use controlled crosses and meiosis to connect a genotype to a phenotype. See Burgess, Powers and Mell, Budding Yeast Saccharomyces cerevisiae as a Model Genetic Organism (2017), pp. 1–2.
The practical value of Saccharomyces cerevisiae as a model organism is the combination of easy laboratory cultivation, accessible genetics, and cellular functions shared with other eukaryotes. A haploid strain has one set of chromosomes, so a changed allele is not accompanied by a second copy at that genetic locus. But a mutation need not produce an observable phenotype under every condition. The yeast is also a whole organism, not a miniature human: transferring a result requires evidence that the relevant function is shared in the target system. See Duina, Miller and Keeney, Budding Yeast for Budding Geneticists (2014): cultivation, genetic tools and conserved functions.
For a concrete example, Hartwell, Culotti and Reid's 1970 work followed temperature-sensitive Saccharomyces cerevisiae strains with successive microscope photographs. Failure to complete a particular part of the cell cycle helped identify required gene functions. Their distinction between when a function is required and where a cell finally stops is especially instructive: the visible endpoint need not be the time of the underlying defect. See Hartwell, Culotti and Reid, Genetic control of the cell-division cycle in yeast. I. Detection of mutants (1970): primary abstract. This is a useful way to turn an observable change in a biological cell into a question about genes and causal order.
In alcoholic fermentation, Saccharomyces cerevisiae converts sugars into ethanol and carbon dioxide. The carbon dioxide helps dough rise; the ethanol is useful in alcoholic drinks. The metabolism also supports production of ATP, a usable cellular energy carrier. This is one metabolic ability of one species, not the definition of every yeast. See Clark, Douglas and Choi, Biology 2e, 7.5: alcohol fermentation and the Burgess, Powers and Mell account above.
For glucose, the ideal net stoichiometry isOne molecule of glucose supplies six carbon chemical atoms: four end up in the two ethanol molecules and two in the two carbon dioxide molecules. The twelve hydrogen and six oxygen chemical atoms also balance. This is a net material balance across several enzyme-catalyzed steps, not a single chemical reaction step or the complete bookkeeping for cellular energy carriers. The standard pathway accounting yields a net two ATP per glucose: the initial breakdown produces the ATP, while the later conversion to ethanol regenerates a coenzyme needed to keep the breakdown going. See Clark, Douglas and Choi, Biology 2e, 7.2: net ATP accounting and the section 7.5 cited above.
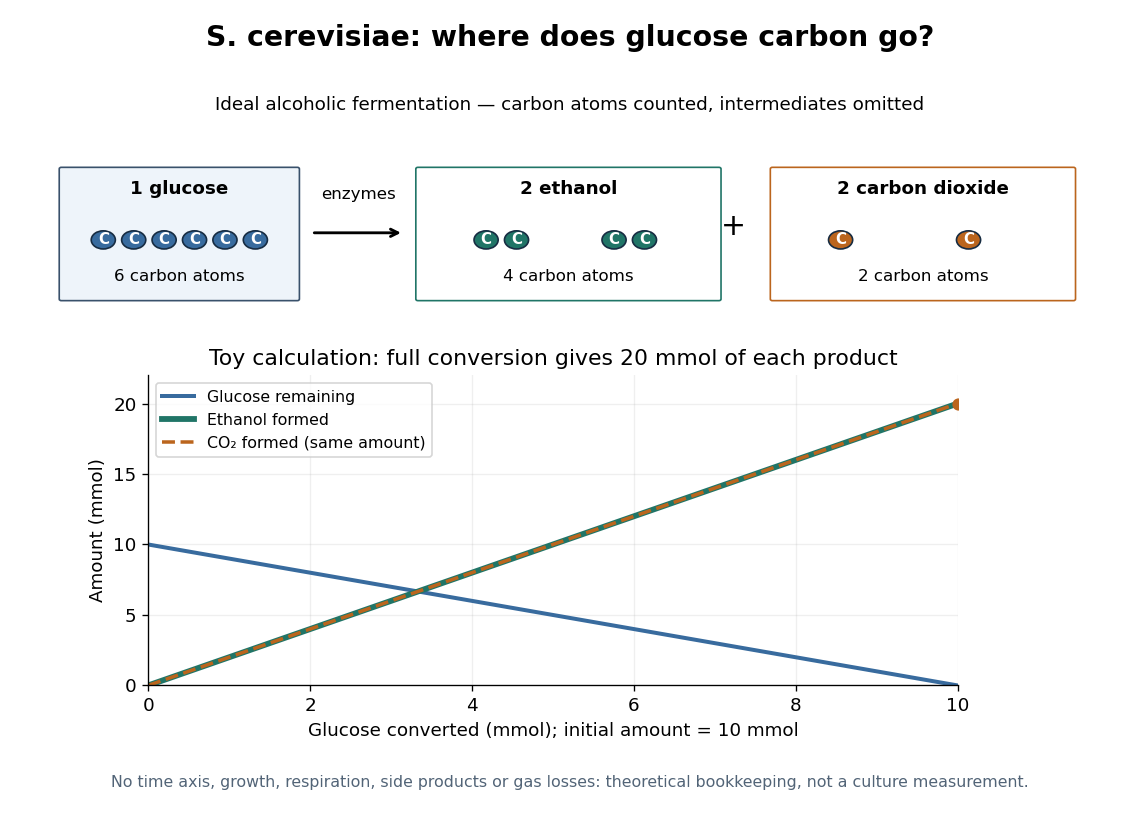
At complete conversion, this toy gives of ethanol and of carbon dioxide. The carbon balance is of carbon chemical atoms. A real culture also builds cellular material, can use other metabolic routes, and may retain dissolved carbon dioxide; the toy is a reference balance rather than a prediction of collected gas or beverage yield.
Although alcoholic fermentation does not require molecular oxygen as a reactant, the presence of molecular oxygen does not force Saccharomyces cerevisiae to stop fermenting. De Deken's 1966 experiments reported predominantly fermentative glucose use during exponential growth in air. Consequently, bubbles do not establish either absence of molecular oxygen or an exclusively fermentative metabolism. See De Deken, The Crabtree Effect: A Regulatory System in Yeast (1966): primary abstract.
Plants are eukaryotes. A typical photosynthetic leaf cell has a cell nucleus, mitochondria, chloroplasts, and a cell wall outside its cell membrane. A root cell need not have chloroplasts; the plant's parts specialize for different functions. Plants perform cellular respiration as well as photosynthesis. See OpenStax Biology 2e, 4.3: plant cell organization.
Articles were limited to the first 100 out of 566 total.



