For an assay begun by mixing free enzyme and substrate, take . The complex has not yet formed and no product has been made. The later small-enzyme limit assumes . Other preincubation protocols could require nonzero initial complex, but these initial conditions are the ones used by the stated inner solution.
Mass action givesThus and are conserved. Eliminating free enzyme yields the stated two-equation system.
With , and , substitution givesThe dimensionless initial data are . The parameter named here is an enzyme kinetic coefficient and is unrelated to the loss parameter used in the later blood-cell question.
Set , , and . On fast time ,For , leading substrate remains . The initial complex buildup therefore solves , , givingTime belongs inside the exponential. Its placement outside the exponential bracket in the printed expression is a typographical error; the derived form satisfies both the kinetic equation and zero initial complex concentration.
Use the longer scale and . The equations becomeAt leading order the fast complex variable has equilibrated to the quasi-steady manifold. ThereforeMatching from the initial layer gives for this outer problem; its implicit solution is . The dimensional substrate loss is the Michaelis-Menten rate with maximum rate and Michaelis constant .
The fast scale resolves the rapid complex buildup that is compressed into a thin initial layer on the substrate-depletion scale. The outer scale follows depletion over a much longer time and cannot satisfy by itself.
In the overlap , the inner solution tends to . The outer solution as has the same limit. Subtracting this common part produces a leading composite approximation,It satisfies the leading initial values and tends to the outer quasi-steady solution after the initial layer. Corrections of order describe the small substrate loss during complex buildup.
In physical concentration coordinates, the two nullclines areSince , the substrate nullcline lies above the complex nullcline for . Starting at , the complex rises and substrate falls; with , this fast segment is nearly vertical when the axes use their respective concentration scales. The trajectory then follows the complex quasi-steady manifold toward the origin. On its slow descending portion it is slightly above the complex nullcline so that ; the leading outer curve itself sets that derivative to zero only at zeroth order.
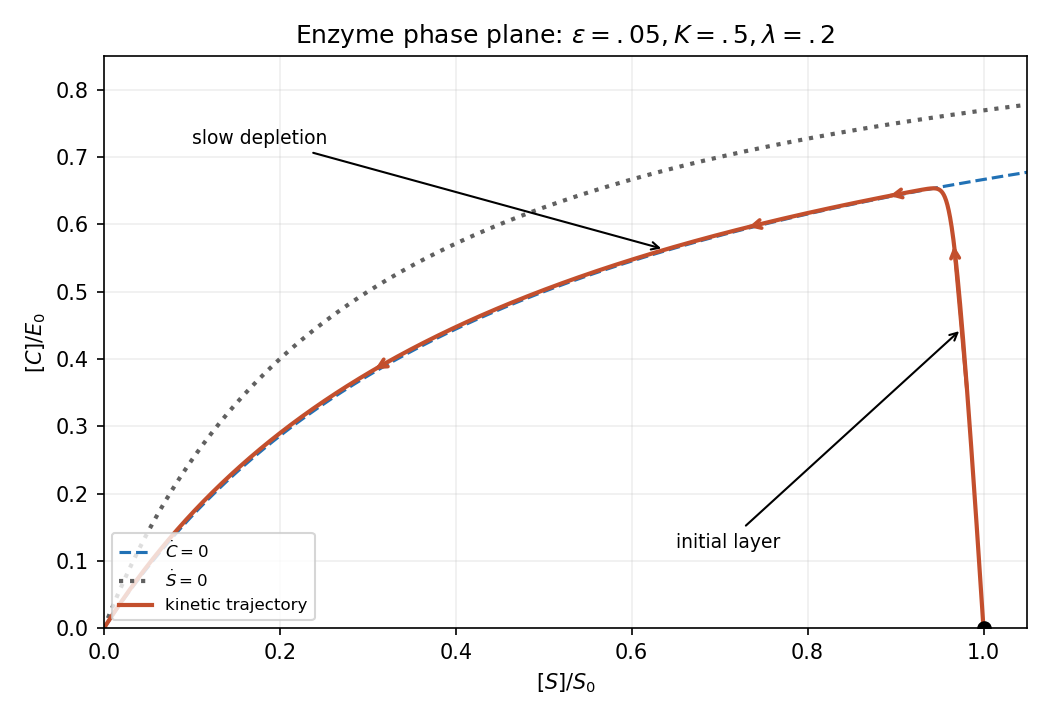
Enzyme kinetics in scaled concentration coordinates: rapid complex buildup followed by slow substrate depletion
. Details. 
The official Oxford course archive advertises an answer for this entire question. Its introductory ask and all seven leaves are covered externally and are not re-solved here.
The decreasing production term represents negative feedback: low red-cell abundance stimulates production, whereas high abundance suppresses it. The linear loss term models removal at constant per-cell rate. SetThen , with . On the physical half-line , decreases from one to zero while increases from zero to infinity. Their unique intersection is the steady state. Its linear derivative is , so it is asymptotically stable.
For small , the intersection lies at large , where ; for large it lies at small , where . HenceImplicit differentiation of gives . The plot joins these two decreasing asymptotic regimes.
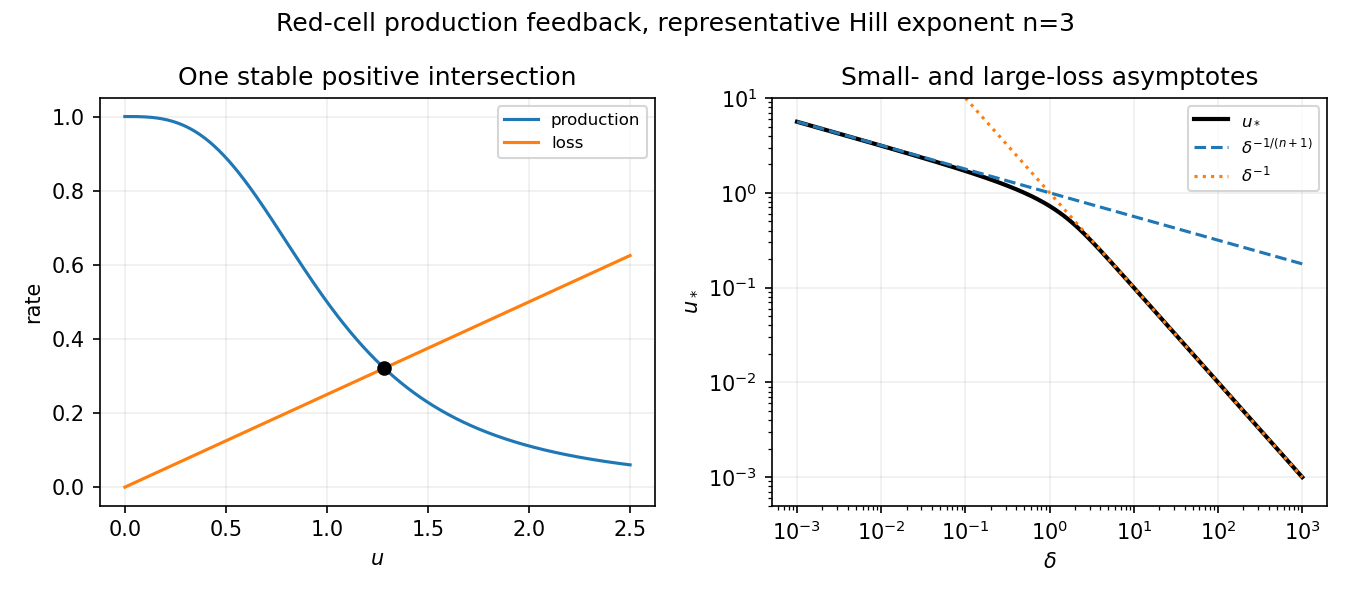
Negative production feedback gives one stable red-cell equilibrium and two limiting concentration scalings
. Details. 
The delay represents the time between feedback sensing and the appearance of newly produced mature cells. In dimensionless time it is , so the equation becomesIt requires a nonnegative initial history on , not just one initial value. Its constant equilibrium is unchanged. Put . A small perturbation obeys , whose characteristic equation isThere is no real root with , because all three terms would have positive sum; zero is never a root either. Starting from the stable zero-delay case, loss of linear stability can therefore occur only when a complex conjugate pair crosses the imaginary axis at a nonzero frequency, the linear signature of a Hopf bifurcation.
For completeness, substituting gives and . Such a crossing requires , withThe first crossing is transversal: . If , the magnitude relation rules out roots in the closed right half-plane for every delay. A nondegenerate nonlinear Hopf conclusion additionally uses the usual bifurcation hypotheses. This is delayed negative feedback in red-cell production.
Resting cells enter proliferation at rate . A proliferating cell takes a fixed cycle time to divide and survives that cycle with probability under a constant death hazard . Thus exit from the proliferating compartment at time is , and it returns twice as many daughter cells to the resting population. Resting-cell loss at rate is separate.
More explicitly, the number currently in the proliferating stage isfor a consistent initial history. Differentiation gives the stated equation. Counting resting-cell entry, loss and daughter-cell return gives its equation. Negative feedback in suppresses recruitment when the resting population is high; its Hill exponent gives a steep response around the concentration scale .
Set and defineThen , so the resting-cell equation becomes exactlyThe nonzero steady state solves , or for positive . The latter right side decreases strictly from to zero. Thus when there is exactly one positive equilibrium,Zero is also an equilibrium; negative populations are outside the biological domain. The same result is visible by intersecting the line with the hump-shaped .
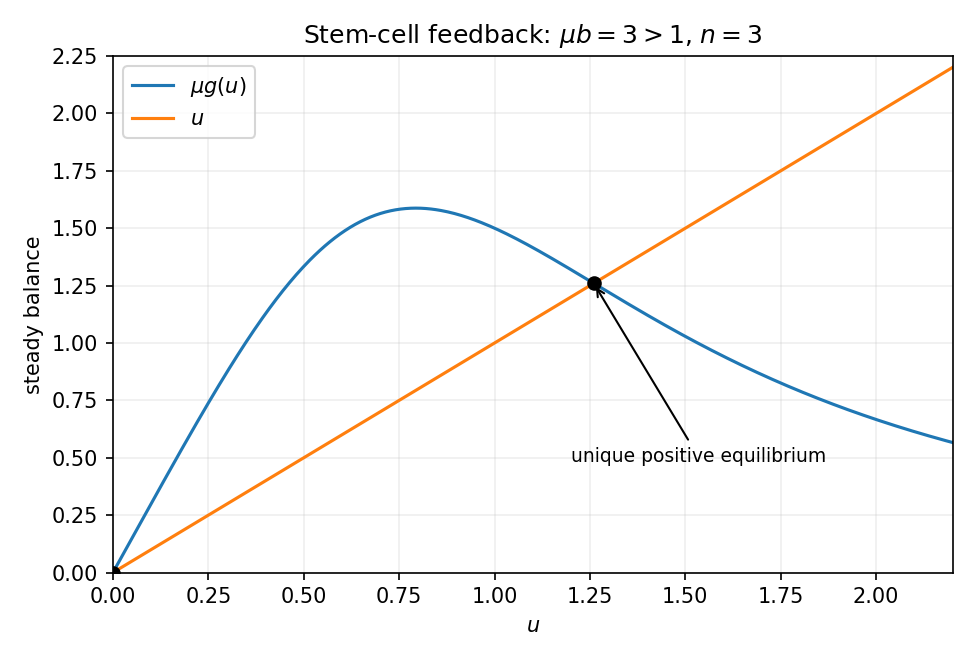
Resting-cell recruitment feedback has one positive equilibrium when the small-population reproduction factor exceeds one
. Details. 
Put . Linearization and a mode giveHere is the coefficient called in the source's characteristic equation; it is not the proliferating-cell death hazard. Any characteristic root with positive real part makes the equilibrium linearly unstable. A nonzero imaginary crossing satisfies and ; these are its Hopf conditions, subject to nondegeneracy.
On slow time , the unit delay becomes . Taylor expansion gives . Dividing the equation by therefore yieldsThis approximation requires slow smooth variation and a denominator bounded away from zero; a vanishing denominator marks failure of this slow reduction. On the fast time , omit only the explicit order- terms, retaining the finite delay:Replacing the delayed argument by the present value on that fast scale would incorrectly erase the dynamics. These are the slow and fast limits of a delayed stem-cell model.
Articles by others on the same topic
There are currently no matching articles.