Spatial summation combines inputs arriving at different synapses. Location matters because a dendrite has axial electrical resistance and leaky membrane capacitance: a local synaptic potential need not arrive at the soma with its original amplitude or time course. A passive dendritic cable makes this attenuation explicit. The superposition principle applies to fixed electric current inputs in a linear passive model, but adding synaptic conductances changes the model's coefficients. Compare voltage changes relative to the same baseline, rather than adding absolute membrane potentials.

A motivating experiment. A 2004 study used – cortical slices from –-day-old rats at –. Somatic whole-cell recordings measured EPSPs in layer-5 pyramidal neurons. Two fine stimulating electrodes were positioned beside imaged dendrites; calcium-sensitive dye localized activation. Each site was stimulated alone, then both together, usually with paired pulses apart. Comparing the combined voltage trace with the sum of individual changes tested the summation rule. Nearby inputs on one branch showed strong amplification at intermediate strengths; inputs on different branches were approximately linear.[ref]
Computational subunits in thin dendrites of pyramidal cells by Alon Polsky and others. pp. 622–623, Figures 1–2; p. 626, Methods
Blocking both excitatory receptor classes eliminated voltage and calcium responses, checking against direct electrical activation. NMDA receptor blockers eliminated or markedly reduced amplification; comparisons with inhibition intact and blocked addressed inhibitory contributions. These controls support local active integration. Passing axons could still recruit unintended synapses; somatic voltage does not measure every local membrane potential. The study tested subthreshold slice responses and pairs of branches, not arbitrary activity in an intact brain.[ref]
Computational subunits in thin dendrites of pyramidal cells by Alon Polsky and others. pp. 622–624: controls; pp. 625–626: limitations
A passive dendritic cable models a uniform dendrite with axial electrical resistance, membrane leak and membrane capacitance, excluding active ion channels. Let be axial electrical resistance per length, membrane electrical resistance times length, and membrane capacitance per length. For voltage deviation from the leak reversal potential, electric charge conservation gives the partial differential equation is imposed inward electric current per length. Units are , and , so is a time and a length. On a source-free semi-infinite cable with imposed and as , the steady state isDifferentiate twice to verify the ordinary differential equation . At , the amplitude is of the boundary amplitude. This is a stationary attenuation law, not the complete waveform of a brief EPSP. Transient passive spread also broadens and delays responses. Finite ends, branch points and the soma's load alter the solution; distance alone cannot specify every real synaptic potential.[ref]
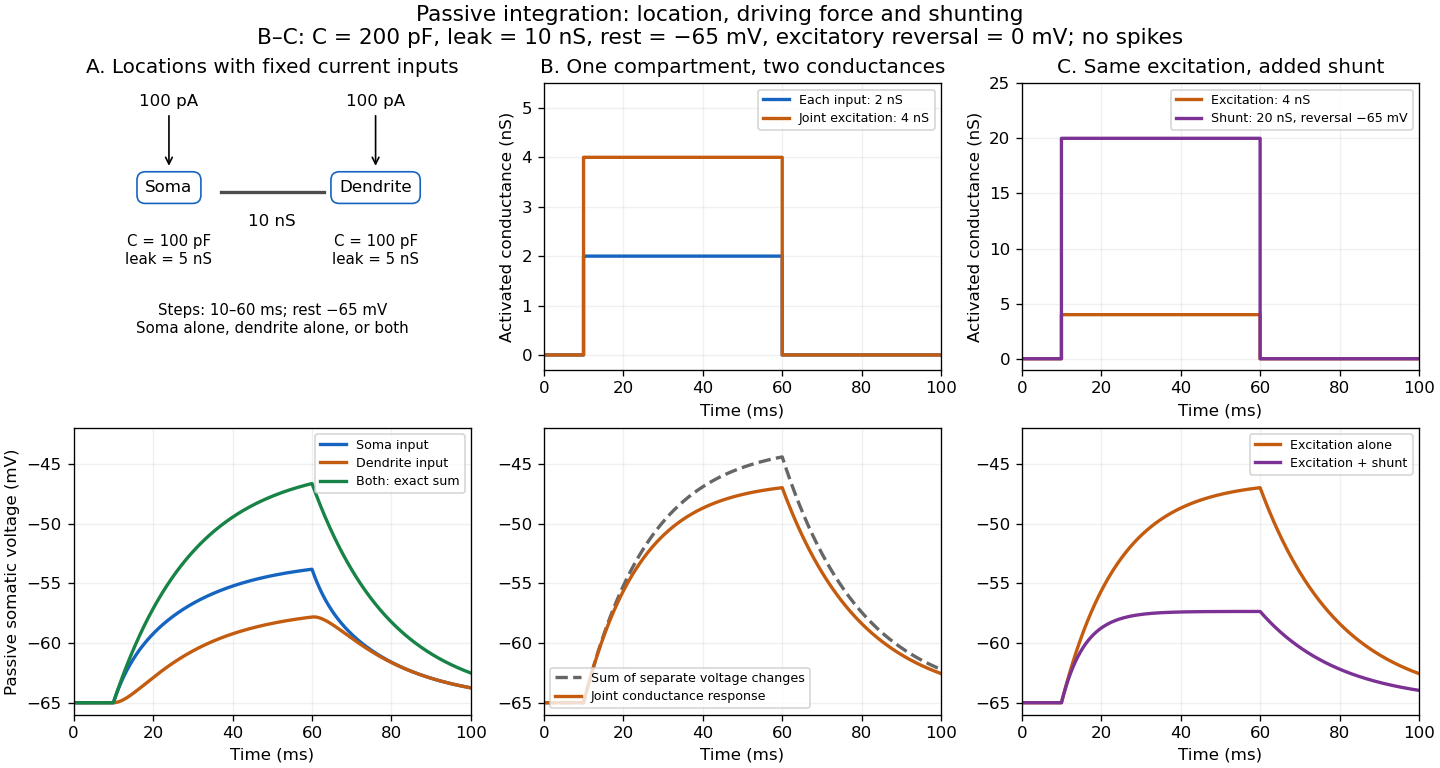
The spatial panel uses two compartments with membrane potentials , one representing the soma and one a dendrite. Set , , with leak reversal potential , each membrane capacitance , each leak electrical conductance and axial electrical conductance . Electric charge conservation givesThis chosen passive model has two decay time constants, for the equal-voltage mode and for the voltage-difference mode. Starting from rest, a step into the soma gives, with the time since onset,while the same step into the dendrite gives is expressed in . Their long-time rises are and respectively. Applying both inputs gives exactly: spatial attenuation coexists with linear summation of prescribed electric currents. After the steps end, both modes decay with their respective time constants. This deliberately coarse model is not a reconstructed dendrite or a fit to the experiment above.
The conductance panels use the existing one-compartment synaptic potential equation, with , , and excitatory reversal potential . For a constant excitatory synaptic conductance , the steady state voltage rise and membrane time constant areEach isolated input has a limiting rise . Adding those isolated rises predicts , but opening both together gives . The two conductances share a changing driving force. This is sublinear input summation even though the voltage ordinary differential equation is linear for each prescribed conductance waveform.
Add with reversal potential to the joint excitation. The limiting rise becomes and the membrane time constant becomes . The shunt alone leaves rest unchanged. At the joint-excitation-only steady state , however, its inward electric current would be : it opposes that excursion. The finite traces in the diagram approach, but need not reach, these limiting voltages. See shunting inhibition for the constant-electric current comparison.
Articles by others on the same topic
There are currently no matching articles.