Topics (374k) Articles (387k) Users (410) Discussions (242) Comments (383) Files (12k) New article
University Physics Volume 3 by Samuel J. Ling and others 10.3 Radioactive Decay by  Codex 0 2026-10-18
A trypsin colorimetric assay follows enzyme activity through absorbance at . Trypsin cleaves an amide bond in the synthetic arginine derivative BAPNA, releasing p-Nitroaniline.[ref]
Enzymatic Assay of APROTININ - Sigma Quality Control Test Procedure. Enzymatic Assay of APROTININ, Sigma quality-control procedure, p. 1: Principle and Conditions
The inspected Sigma procedure prepares fresh trypsin in cold hydrochloric acid and fully dissolves BAPNA. Its buffer solution stock contains triethanolamine and calcium chloride, at pH . Three cuvettes compare trypsin, trypsin plus the enzyme inhibitor aprotinin, and a blank replacing trypsin with its acid solvent. Sodium chloride solution replaces aprotinin in the uninhibited control. A thermostatted instrument for spectrophotometry holds and a light path. After equilibration, adding BAPNA starts approximately five minutes of absorbance recording. The uninhibited sample checks activity; the blank checks background; the inhibited sample tests suppression.[ref]
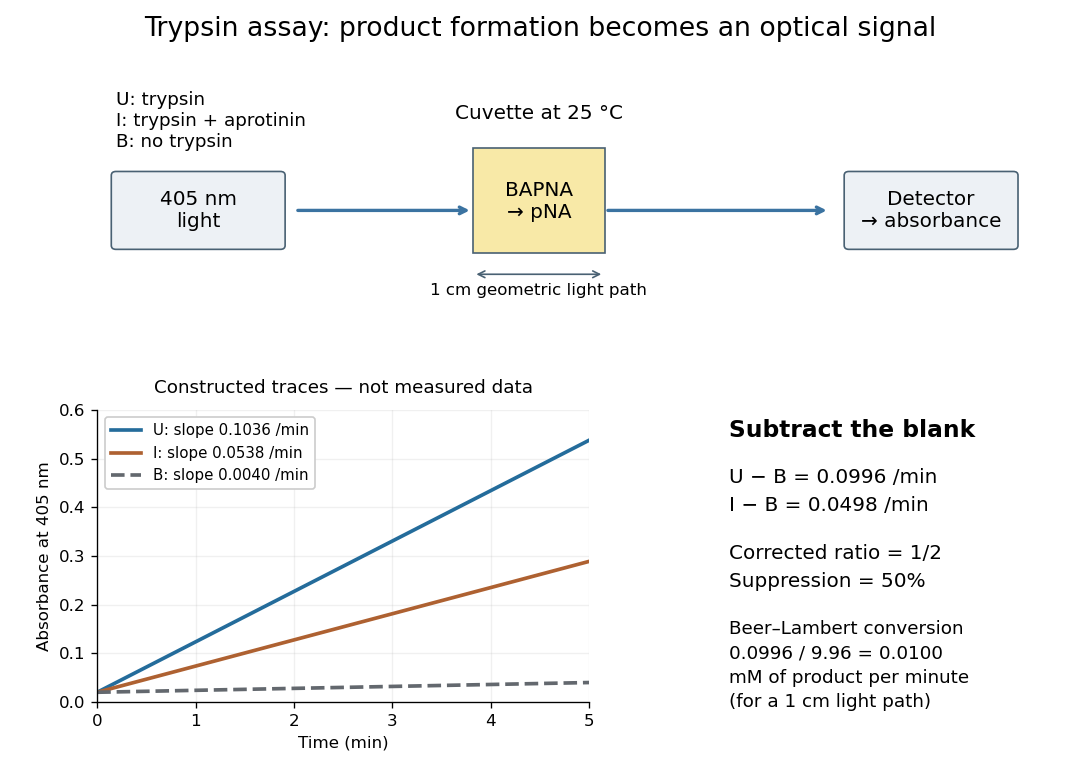
Let , and denote the measured absorbance slopes per minute over the same linear time interval. Blank subtraction gives and . If p-Nitroaniline accounts for the changing absorbance, the Beer-Lambert law givesHere is product molar concentration and is the geometric light path through the chemical solution. Sigma uses .[ref]
Enzymatic Assay of APROTININ - Sigma Quality Control Test Procedure. Enzymatic Assay of APROTININ, p. 2: Calculations, millimolar extinction coefficient at 405 nm
Choose original illustrative slopes , and . The corrected uninhibited slope is , giving at . In , the product amount of substance increases at . The corrected inhibited slope is , half as large. The relative suppression is thereforeThe background cancels in the numerator, but remains essential in the denominator. Using uncorrected slopes would instead give about . Differentiating with fixed and explains the rate conversion; dimensional analysis checks it independently, since .
The inference is a reaction rate on BAPNA under the stated conditions, rather than a direct count of trypsin molecules or proof of every cut in a protein. Cloudiness, other absorbing solutes, or different product protonation can compromise the Beer-Lambert law interpretation. A matched blank and a linear interval are therefore part of the measurement's meaning. A coloured enzyme inhibitor may require its own matched blank; a changed substrate or pH requires a fresh calibration. The constructed constant slopes above describe only that interval, not indefinite product accumulation.
Write a peptide's protein primary structure from its N-terminus toward its C-terminus. The usual simplified trypsin cleavage specificity rule places a cut immediately after K (lysine) or R (arginine), unless the next amino acid residue is P (proline). The following amino acid residue is essential: a terminal K or R has no following peptide bond to cut. The inspected institutional documentation describes proline as usually blocking cleavage, and explicitly lists sequence contexts in which that blocking is negligible. It also warns that experimental results can differ from sequence-based predictions. Thus “never before proline” is too strong.[ref]
For an original worked example, stipulate complete cleavage at all sites allowed by that simplified rule in the twelve-amino acid residue sequenceA denotes alanine, G denotes glycine, and K, R and P have the meanings above. Cuts follow positions , and . Position is R, but its following P suppresses that cut in the stipulated rule; position is terminal K. Notice that the R in ARPK is retained inside the fragment, despite being a usually favoured trypsin target.
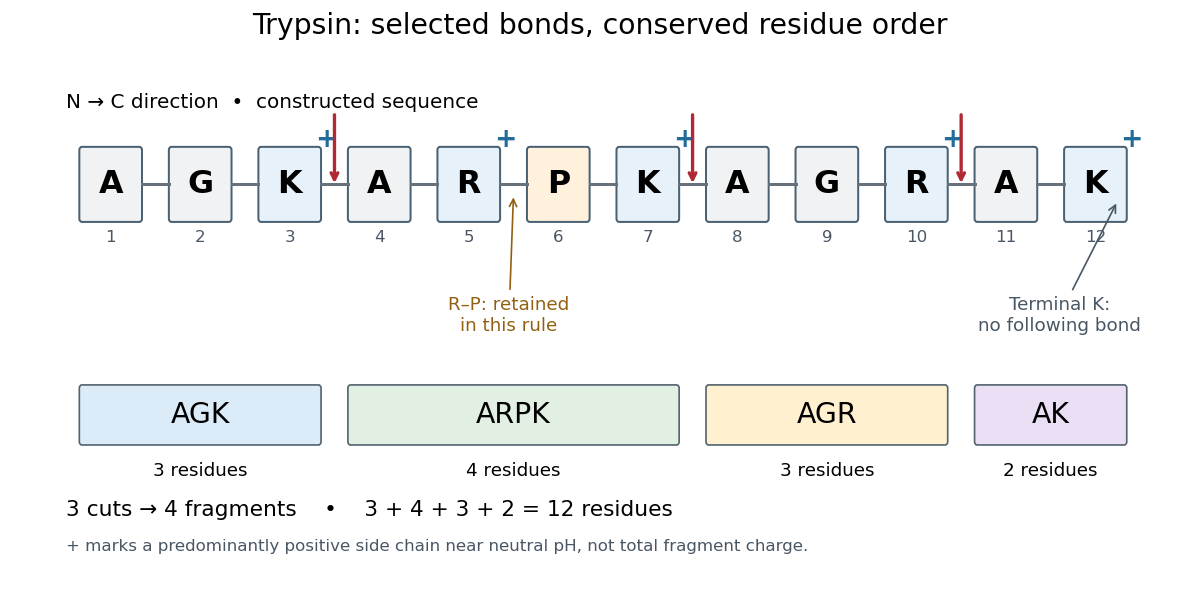
Trypsin cleavage specificity: three selected cuts make four peptide fragments
. Original sequence and prediction under the simplified K/R rule with suppression before proline. Blue plus signs identify predominantly positive lysine and arginine amino acid side chains near neutral pH, not the net electric charge of each fragment. The example is constructed, not an observed digest. Details.Near neutral pH, the lysine and arginine amino acid side chains undergo predominant protonation and carry positive electric charge. This helps distinguish those amino acid residues from the uncharged letter symbols used to write the sequence; those symbols specify identities, not whole-fragment electric charges.[ref]
26.1 Structures of Amino Acids. Organic Chemistry by John McMurry; Table 26.1, lysine and arginine rows; concluding classification paragraph, side-chain protonation at pH 7.3
Fragment accounting checks the prediction: lengths conserve the twelve amino acid residues. The original linear chain has eleven peptide bonds; the four fragments retain , so three were hydrolysed. Three water molecules are consumed per original chain in this formal stoichiometry. More generally, cutting distinct bonds of one linear peptide makes fragments: each cut splits one connected piece into two. This argument assumes an unbranched chain without additional links joining the pieces.
A missed trypsin cleavage at position would instead give , merging two neighbouring fragments without changing their order. Even a correct cleavage preference does not guarantee complete proteolysis; predicted fragment boundaries describe a model, while actual boundaries require evidence from the digest.
Pinned article: Introduction to the OurBigBook Project
Welcome to the OurBigBook Project! Our goal is to create the perfect publishing platform for STEM subjects, and get university-level students to write the best free STEM tutorials ever.
Everyone is welcome to create an account and play with the site: ourbigbook.com/go/register. We belive that students themselves can write amazing tutorials, but teachers are welcome too. You can write about anything you want, it doesn't have to be STEM or even educational. Silly test content is very welcome and you won't be penalized in any way. Just keep it legal!
Intro to OurBigBook
. Source. We have two killer features:
- topics: topics group articles by different users with the same title, e.g. here is the topic for the "Fundamental Theorem of Calculus" ourbigbook.com/go/topic/fundamental-theorem-of-calculusArticles of different users are sorted by upvote within each article page. This feature is a bit like:
- a Wikipedia where each user can have their own version of each article
- a Q&A website like Stack Overflow, where multiple people can give their views on a given topic, and the best ones are sorted by upvote. Except you don't need to wait for someone to ask first, and any topic goes, no matter how narrow or broad
This feature makes it possible for readers to find better explanations of any topic created by other writers. And it allows writers to create an explanation in a place that readers might actually find it.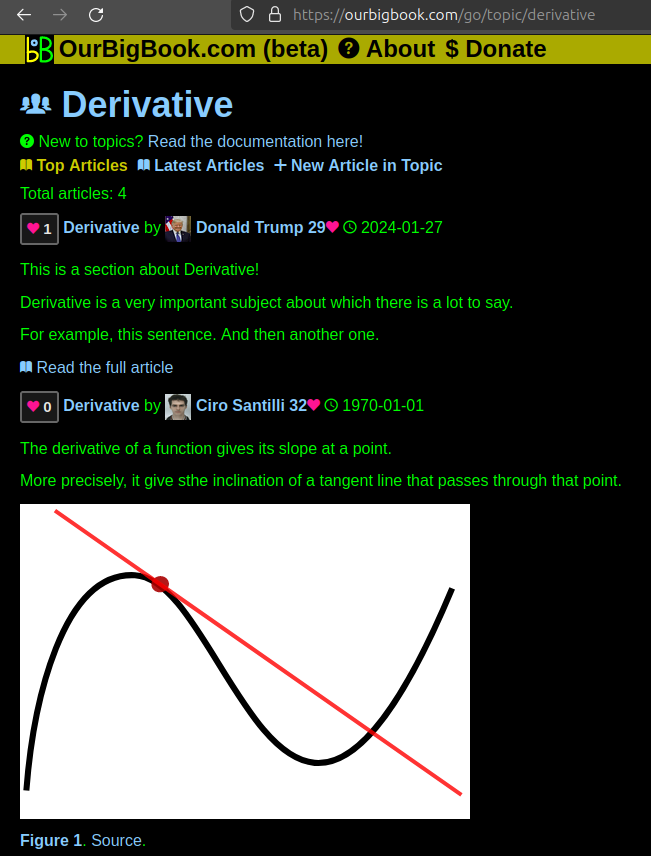
Figure 1. Screenshot of the "Derivative" topic page. View it live at: ourbigbook.com/go/topic/derivativeVideo 2. OurBigBook Web topics demo. Source. - local editing: you can store all your personal knowledge base content locally in a plaintext markup format that can be edited locally and published either:This way you can be sure that even if OurBigBook.com were to go down one day (which we have no plans to do as it is quite cheap to host!), your content will still be perfectly readable as a static site.
- to OurBigBook.com to get awesome multi-user features like topics and likes
- as HTML files to a static website, which you can host yourself for free on many external providers like GitHub Pages, and remain in full control
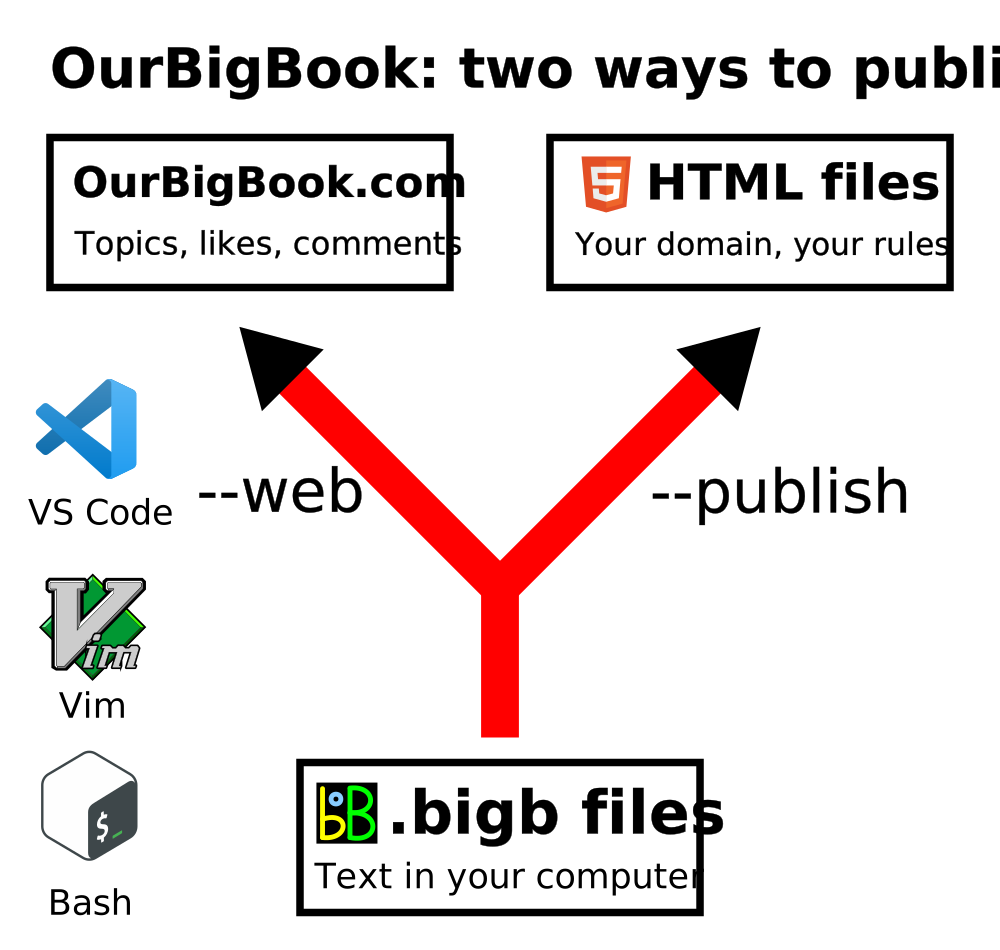
Figure 2. You can publish local OurBigBook lightweight markup files to either OurBigBook.com or as a static website.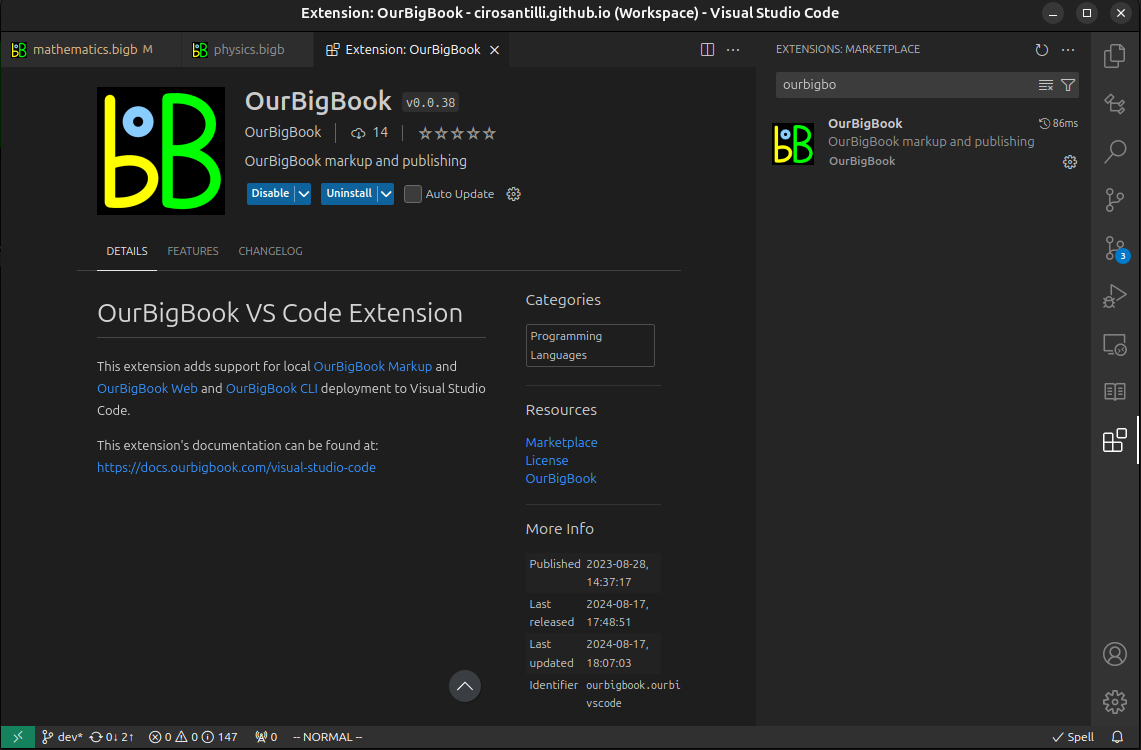
Figure 3. Visual Studio Code extension installation.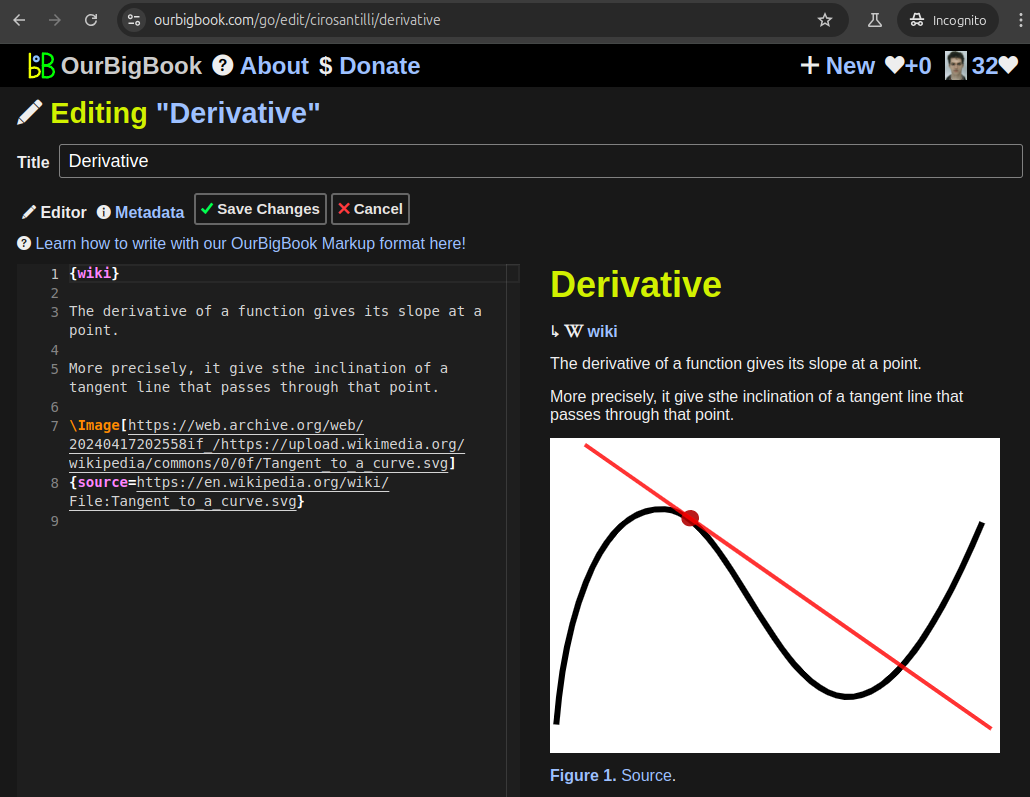
Figure 5. . You can also edit articles on the Web editor without installing anything locally. Video 3. Edit locally and publish demo. Source. This shows editing OurBigBook Markup and publishing it using the Visual Studio Code extension. 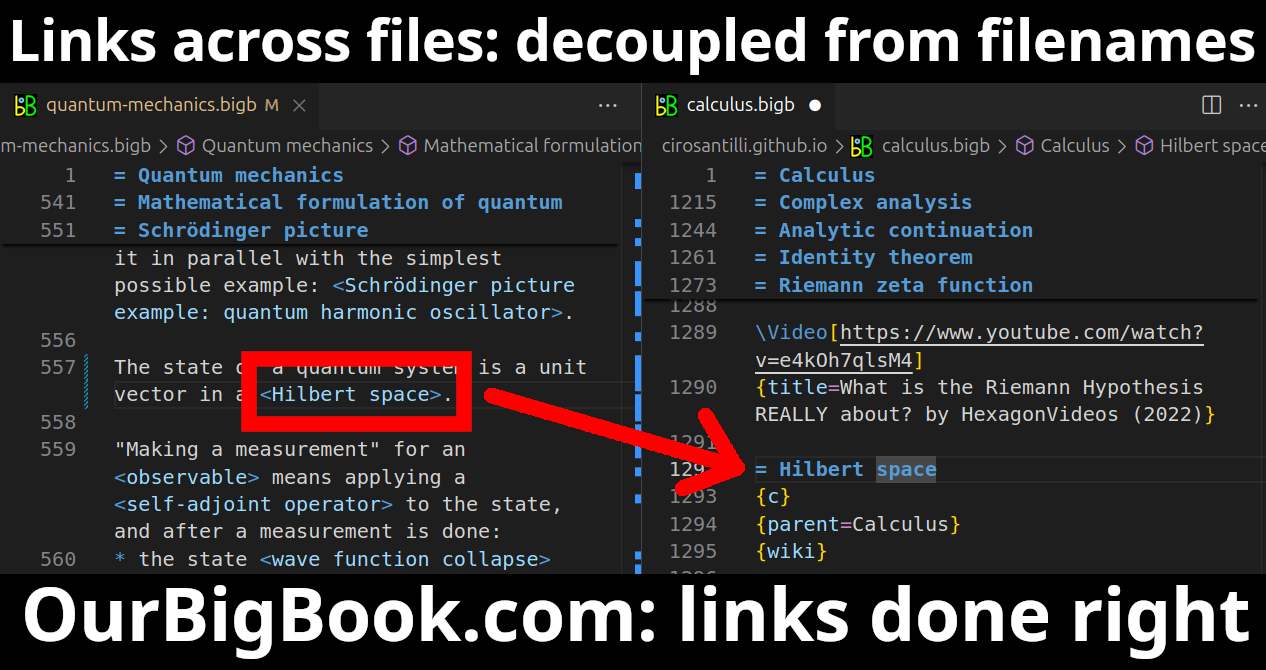
- Infinitely deep tables of contents:
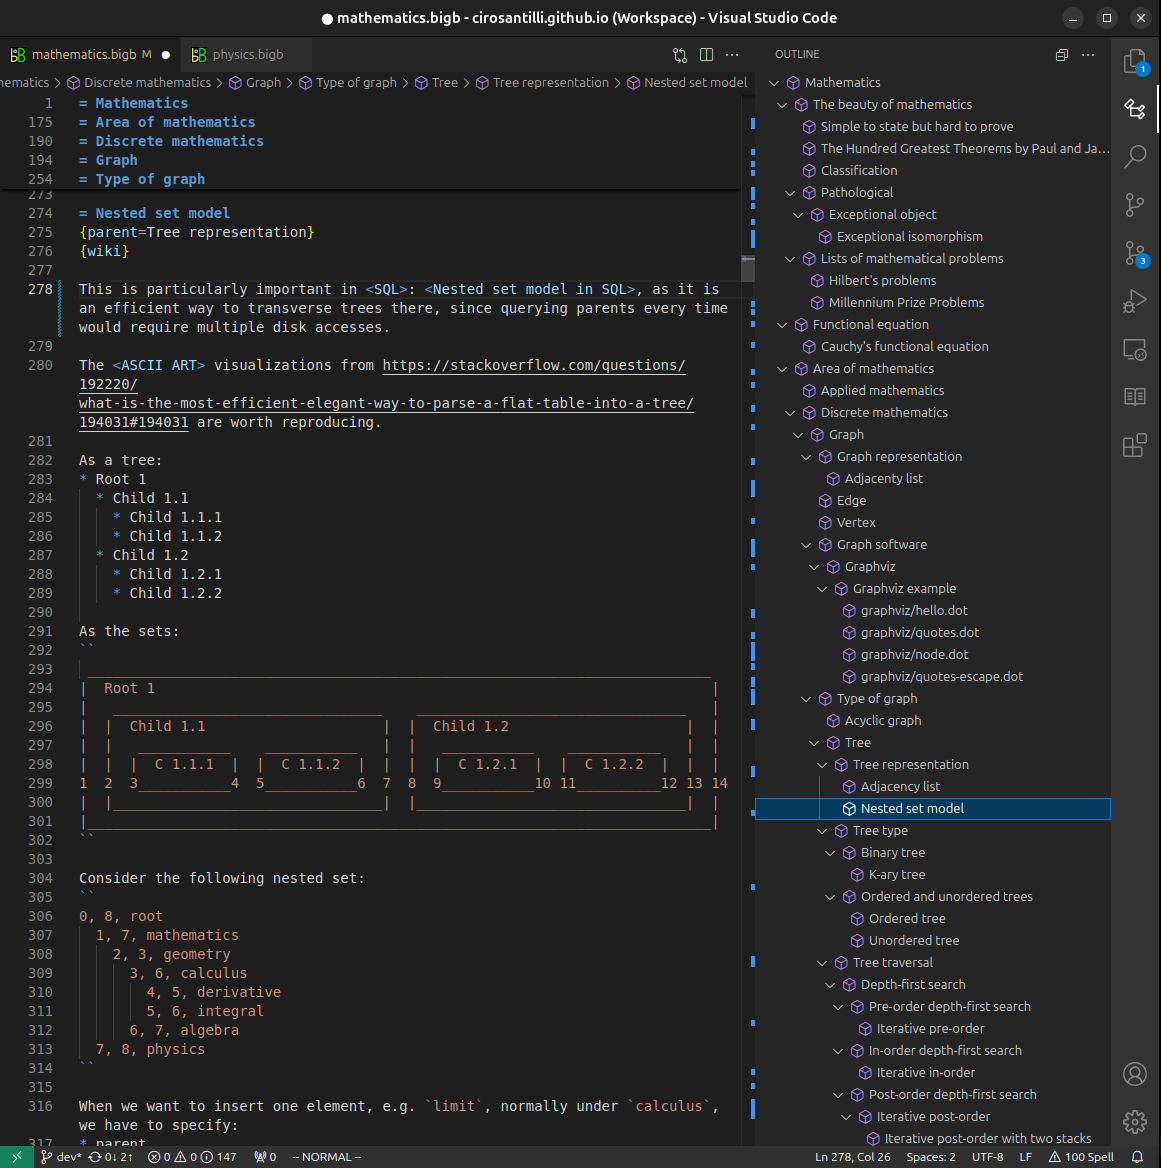


All our software is open source and hosted at: github.com/ourbigbook/ourbigbook
Further documentation can be found at: docs.ourbigbook.com
Feel free to reach our to us for any help or suggestions: docs.ourbigbook.com/#contact