The Golgi apparatus modifies and sorts cargo arriving from the endoplasmic reticulum for delivery to other cellular destinations. The eponym refers to Camillo Golgi.
Its usual stacked organization is polarized: cargo enters on the cis side, encounters medial processing regions, and leaves through the trans side and trans-Golgi network. Golgi cisternae enclose a Golgi lumen separated from the surrounding cytosol. Processing changes cargo; sorting selects its destination.[ref]
The Golgi Apparatus. The Cell: A Molecular Approach, 2nd edition by Geoffrey M. Cooper; Organization of the Golgi, Figures 9.22–9.23; Protein Sorting and Export from the Golgi Apparatus
This division of labor explains why reaching the Golgi apparatus does not imply being secreted: cargo can take different onward routes, while resident enzymes continue working there. The conventional route discussed here is part of secretory protein routing; many cytosol proteins never enter it.
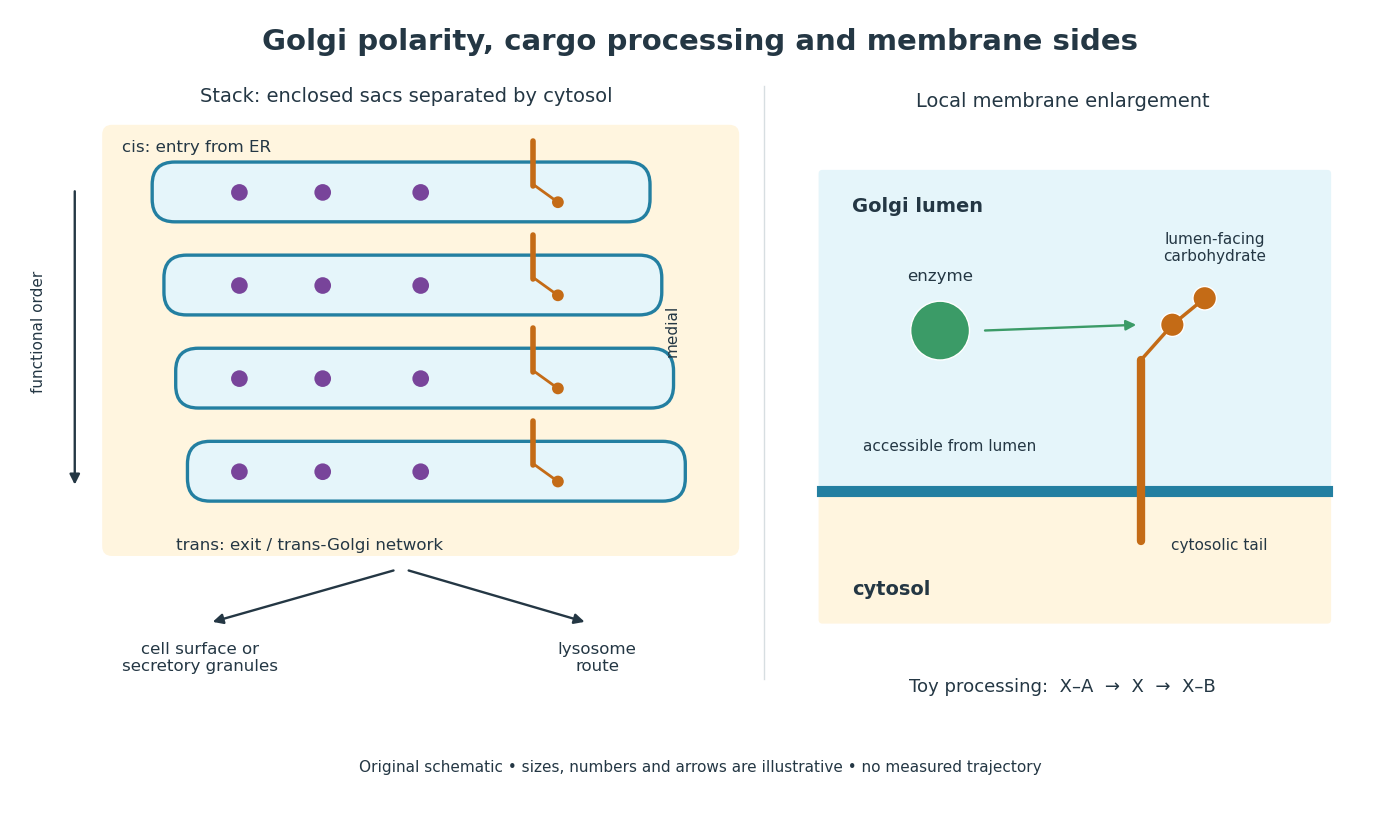
Golgi apparatus polarity, processing and membrane sides
. Original schematic of a stack and a local membrane enlargement. The spaces between Golgi cisternae contain cytosol, while each enclosed sac contains Golgi lumen. Purple cargo is soluble; the orange membrane protein has a lumen-facing carbohydrate chain and a cytosolic tail. Arrows show functional ordering, not a measured trajectory or a universal carrier mechanism. The chain-processing symbols are a constructed example. Details.
A Golgi cisterna is a flattened membrane-enclosed sac. Stacking several sacs does not make their interiors one open space: membrane separates Golgi lumen from intervening cytosol.[ref]
The Golgi Apparatus. The Cell: A Molecular Approach, 2nd edition by Geoffrey M. Cooper; Organization of the Golgi, Figure 9.22: membrane-enclosed cisternae
The Golgi lumen is the enclosed interior of a Golgi cisterna, distinct from the surrounding cytosol.
The membrane-sidedness rule in secretory protein routing still applies within the Golgi apparatus. For a local worked example, stipulate a membrane protein with a carbohydrate chain exposed to Golgi lumen and a tail exposed to cytosol. An enzyme confined to Golgi lumen can contact that chain, but cannot directly contact the cytosolic tail without a boundary-crossing step. A change in which Golgi cisterna contains the protein need not turn the protein over. Thus chemical accessibility and cargo location are different questions: moving cargo onward preserves its membrane sides under the budding and fusion operations described in secretory protein routing.
Golgi cargo processing includes enzyme-mediated remodeling of attached oligosaccharides. Glycosylation can involve addition of sugars, while processing can also remove them. Different Golgi apparatus regions have different processing enzymes; their substrate requirements constrain the order of possible chemical reactions.[ref]
Transport from the ER through the Golgi Apparatus. Molecular Biology of the Cell, 4th edition by Bruce Alberts and others; Oligosaccharide Chains Are Processed in the Golgi Apparatus; The Golgi Cisternae Are Organized as a Series of Processing Compartments, Figure 13-28
An original model makes the importance of ordering explicit. Write a toy carbohydrate chain as , read with its terminal symbol on the right. Define a trimming function that removes a terminal , and an extension function that adds only when the terminal symbol is . In every other case the corresponding function leaves the chain unchanged. ThenIn particular, but : the two functions do not commute. Each result follows by inspecting the terminal symbol before applying the stipulated rule. These symbols are artificial labels, rather than a natural oligosaccharide sequence or measured enzyme pathway. The example explains why “two processing steps occurred” does not determine the product unless their order and substrate conditions are also specified. In the Golgi apparatus, spatial organization can help arrange successive opportunities for processing.
The trans-Golgi network is the sorting and export region at the trans side of the Golgi apparatus. Onward traffic can supply the cell membrane, secretory granules, or the lysosome route.[ref]
The Golgi Apparatus. The Cell: A Molecular Approach, 2nd edition by Geoffrey M. Cooper; Protein Sorting and Export from the Golgi Apparatus, Figure 9.27 and lysosomal targeting discussion
Processing and sorting answer different questions. In a constructed example, two cargo proteins could receive the same carbohydrate modification yet carry different targeting information and leave in different transport vesicles. Conversely, two chemically different cargo proteins could share a destination. A processing readout alone therefore cannot establish the final address; an experiment must also identify cargo location or delivery. Return traffic and retention likewise matter: the Golgi apparatus is a working compartment, not merely a one-way queue that empties all of its enzymes into outgoing carriers.
In cisternal maturation, a cargo-containing Golgi cisterna changes from early to later identity as its resident proteins change; retrieval of resident enzymes toward earlier compartments helps maintain Golgi apparatus polarity. In the contrasting stable-compartment model, cargo moves between persistent Golgi cisternae in transport vesicles. These mechanisms need not be mutually exclusive.[ref]
Transport from the ER through the Golgi Apparatus. Molecular Biology of the Cell, 4th edition by Bruce Alberts and others; Transport Through the Golgi Apparatus May Occur by Vesicular Transport or Cisternal Maturation, Figure 13-30 and concluding comparison
The distinction is between following cargo and following its container. A cargo label encountered first in an early processing environment and later in a late one is compatible with either changing containers or a container changing identity. Finding transport vesicles nearby does not by itself establish which cargo they carry or their direction of travel. Testing cisternal maturation therefore requires evidence about compartment identity and continuity as well as cargo position; a single mechanism should not be assumed for every cargo and biological cell.
The pancreatic secretory-protein pulse-chase experiment of James D. Jamieson and George E. Palade used guinea pig pancreas slices and a short pulse of tritium-labeled leucine followed by a chase. Thin sections on coated grids received Ilford L-4 emulsion; developed grains were read against structures by electron microscopy. Their Table II localized label to peripheral Golgi apparatus vesicles and condensing vacuoles, without significant labeling of the piled flattened Golgi cisternae.[ref]
Intracellular Transport of Secretory Proteins in the Pancreatic Exocrine Cell. II. Transport to Condensing Vacuoles and Zymogen Granules by James D. Jamieson and George E. Palade. p. 598 Methods; p. 609 Table II and its footnote
An important comparison checked the isolated granule fraction by autoradiography and electron microscopy: early labeling came substantially from contaminating condensing vacuoles, rather than mature secretory granules. Thus a fraction's name did not uniquely identify the labeled structure. This supported transport into the Golgi apparatus's condensing region and onward storage, while fixed samples and finite grain localization limited interpretation. It did not establish a resolved cis-to-trans itinerary across every Golgi cisterna. The preparation's labeling also did not mark secretory cargo exclusively.[ref]
Intracellular Transport of Secretory Proteins in the Pancreatic Exocrine Cell. II. Transport to Condensing Vacuoles and Zymogen Granules by James D. Jamieson and George E. Palade. p. 609 Figure 14; p. 613, Transport of Labeled Proteins to Condensing Vacuoles, Zymogen Granules, and the Acinar Lumen: comparison of fraction labeling with microscopy; p. 611, General Premises
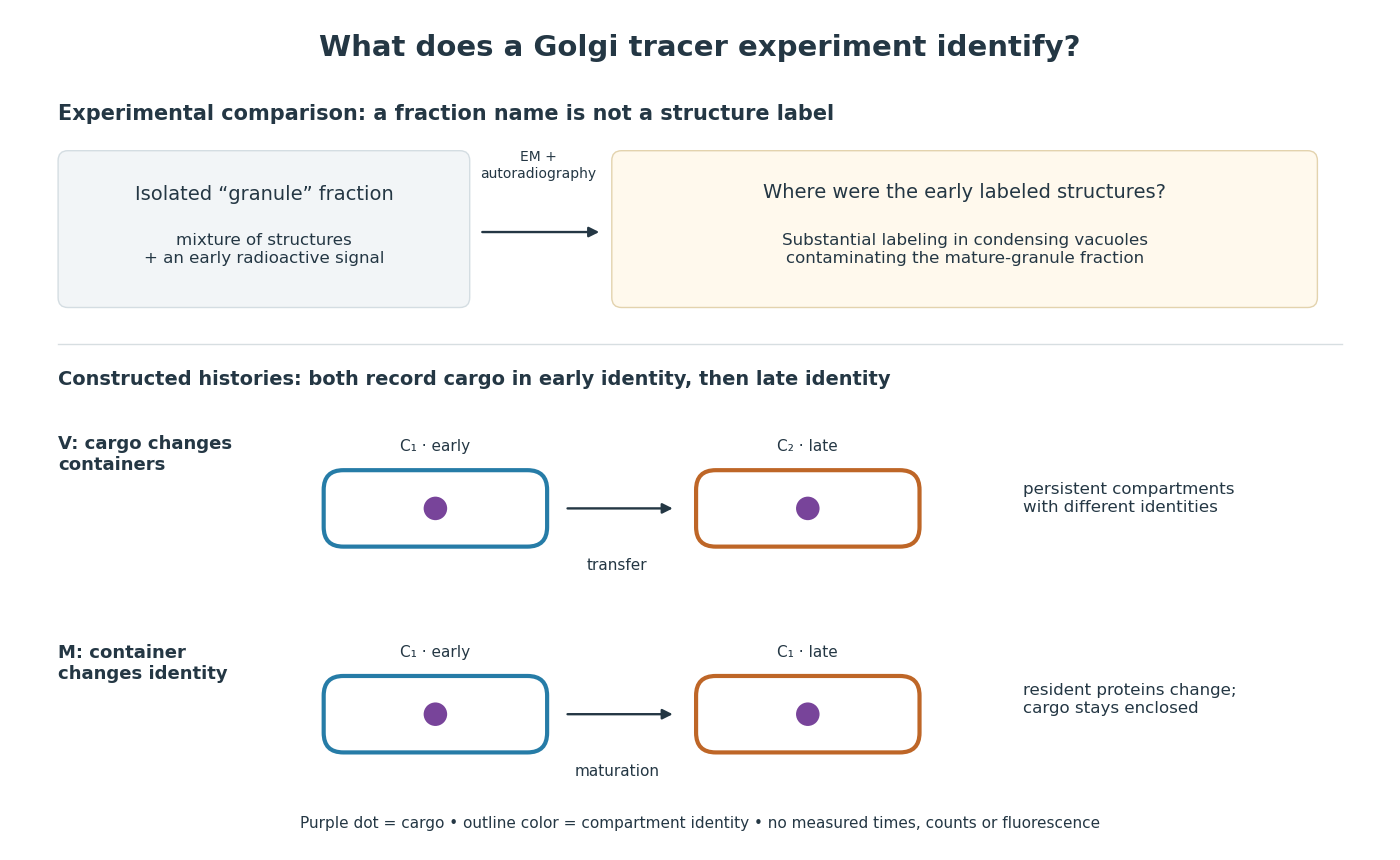

For a minimal worked inference, record only two outcomes for one labeled cargo cohort: early identity first, late identity later. Model V transfers cargo from container to container ; model M keeps it in while changes identity. Both produce the same recorded outcomes, so those outcomes alone cannot distinguish V from M. The proof is constructive: exhibit both histories and discard container identity from each record. More informative tracking would retain both cargo and resident-compartment markers, while resolving whether the same compartment persists. This is why pulse-chase analysis and compartment tracking answer complementary questions about the Golgi apparatus.
Articles by others on the same topic
There are currently no matching articles.