
Deoxyribozyme 2026-11-05
A deoxyribozyme, or DNAzyme, is a DNA molecule with catalytic activity. Its nucleotide sequence permits a functional folded structure that accelerates a specified chemical reaction. Catalytic function is distinct from merely recognizing or binding a target, as an aptamer can do. The term identifies the catalytic material; it does not imply that every DNAzyme catalyzes the same reaction.
A motivating primary experiment by Ronald R. Breaker and Gerald F. Joyce selected DNA molecules that promoted cleavage of an RNA linkage. Their 1994 paper started with a large randomized DNA population and used repeated selection and amplification to enrich activity. The selected catalyst required lead ions under the tested conditions, and an intermolecular version achieved repeated substrate turnover. This established catalytic DNA in a laboratory selection system, rather than demonstrating a naturally occurring cellular enzyme.[ref]
A DNA enzyme that cleaves RNA by Ronald R. Breaker and Gerald F. Joyce. Abstract, Background, Results and Conclusions
A DNAzyme turnover experiment can distinguish a catalyst from a one-use reagent. For a constructed molecular count, suppose a preparation contains active DNA catalyst and produces specifically cleaved product. The ratiomeans ten reactions per active catalyst molecule on average. This interpretation requires controls for uncatalyzed product formation and an appropriate count of active molecules. The ratio alone gives neither a reaction rate nor a turnover number per unit time.
A time-resolved experiment additionally measures initial reaction rates while varying substrate concentration and holding other conditions fixed. A selected sequence, its inactive or altered controls and a substrate-only reference answer different questions about sequence dependence and background cleavage. Yingfu Li and Ronald R. Breaker's primary measurements of chemically driven RNA degradation illustrate why that baseline matters when quantifying catalytic enhancement.[ref]
Kinetics of RNA Degradation by Specific Base Catalysis of Transesterification Involving the 2′-Hydroxyl Group by Yingfu Li and Ronald R. Breaker. Abstract: defined substrates and background cleavage mechanism
A catalyst changes the rate of approach to a chemical equilibrium without supplying unlimited chemical free energy. Its performance depends on folding, molecular recognition, reaction chemistry and product release; observing binding alone does not establish all of these functions.
DNAzyme turnover experiment 2026-11-05
A DNAzyme turnover experiment measures how much reaction product a DNAzyme forms over time relative to the amount of active catalyst. Its central distinction is between one productive event per catalyst molecule and repeated substrate processing. The original deoxyribozyme paper reported an intermolecular catalyst with repeated turnover, rather than merely stable binding to its target.[ref]
A DNA enzyme that cleaves RNA by Ronald R. Breaker and Gerald F. Joyce. Abstract, Results: intermolecular catalytic activity and turnover
The observable should be chemically identified product, for example a resolved cleavage product quantified from an appropriately calibrated gel electrophoresis signal. Record a time course and distinguish the catalyst-dependent contribution from initial product and substrate-only background. An altered-sequence control tests sequence dependence; it does not automatically replace a measurement of background chemistry.
For a constructed example, suppose the initial substrate concentration is and active catalyst concentration is . Background-corrected product reaches after 20 minutes. ThenThe first is a dimensionless cumulative count; the second is an interval-average rate. Neither is automatically the turnover number at saturating substrate. Substrate depletion, changes in active catalyst and product inhibition can make the time course nonlinear.
A rapid initial product burst followed by a slower nearly linear phase can indicate different kinetic stages. For illustration,contains a burst amplitude and later slope . Such a curve motivates investigating DNAzyme product-release limitation, but does not uniquely prove that mechanism: catalyst heterogeneity or inactivation can also alter the trace. Independent perturbations and product-release observations are needed to distinguish explanations.
A background reference matters especially when the substrate can cleave chemically without the DNAzyme. The primary analysis of chemically driven RNA degradation provides the relevant distinction between baseline cleavage and catalytic enhancement.[ref]
Kinetics of RNA Degradation by Specific Base Catalysis of Transesterification Involving the 2′-Hydroxyl Group by Yingfu Li and Ronald R. Breaker. Abstract: background cleavage and interpretation of rate enhancement
RNA degradation 2026-11-05
RNA degradation is the chemical or enzymatic breakdown of RNA, including cleavage of its phosphodiester bonds into shorter strands. Fragmentation can remove the continuity needed for an RNA molecule's function even while much of its nucleotide sequence remains present. Ribonucleases catalyze RNA cleavage; chemical cleavage also occurs without an enzyme.
A chemical route exploits the hydroxyl group at the position of ribose. Its oxygen can act as a nucleophile toward the adjacent backbone phosphorus, producing an internal transesterification that breaks the chain. In their 1999 primary study, Yingfu Li and Ronald R. Breaker used chimeric DNA/RNA substrates to measure hydroxide-dependent cleavage of RNA phosphodiester bonds. Such a substrate isolates a susceptible linkage within a defined molecular context, allowing chemical instability to be measured separately from a complex sample's overall fragmentation pattern.[ref]
Kinetics of RNA Degradation by Specific Base Catalysis of Transesterification Involving the 2′-Hydroxyl Group by Yingfu Li and Ronald R. Breaker. Abstract and p. 5364: substrates and internal phosphoester-transfer mechanism
An illustrative kinetic model follows the number of molecules that remain intact under constant conditions. If each intact molecule has a constant probability per unit time of undergoing its first destructive cleavage, thenThe last quantity is an RNA half-life in this model. With stipulated , half the starting molecules remain intact after about , and after an hour. The numerical rate is an example, not a universal value for RNA or a measurement from the cited experiment.
A cleavage need not remove material from the tube: breaking one long RNA into two pieces initially preserves its total number of nucleotides. Consequently a concentration measurement can stay almost unchanged while RNA integrity declines. An electropherogram can reveal redistribution toward shorter fragments, while a short target region may remain detectable by reverse transcription and polymerase chain reaction. The relevant question is which molecular continuity the intended assay requires.
Ronald R. Breaker 2026-11-05
Ronald R. Breaker is a biochemist at Yale University whose research investigates catalytic and regulatory functions of nucleic acids. His university biography connects his laboratory's work on deoxyribozymes with its investigations of riboswitches, in which RNA recognizes a molecular signal and affects gene expression.[ref]
Ronald Breaker profile at Yale School of Medicine. Biography: catalytic DNA and metabolite-binding messenger RNA
In the 1994 primary paper with Gerald F. Joyce, Breaker reported a DNA catalyst that cleaves an RNA linkage. The experiment used in vitro selection: molecules with useful activity were enriched through successive selection and amplification rounds. The selected chemistry depended on lead ions, so the result established catalytic capacity under the tested conditions, not the existence of a natural cellular DNA enzyme.[ref]
A DNA enzyme that cleaves RNA by Ronald R. Breaker and Gerald F. Joyce. Abstract, Background, Results and Conclusions
The paper's intermolecular catalyst had a reported turnover number of about . An original counting example explains the term: if of active catalyst each process one substrate per minute under sustained substrate-saturating conditions, the initial production rate is approximately . The catalyst can process more than its own molecular count over successive cycles. This differs from a reagent consumed once per cleavage. Binding, chemical reaction and product release can impose different kinetic limits.
Breaker later coauthored with Yingfu Li the primary study of chemically driven RNA degradation. That work supplies a baseline for interpreting catalysis: an apparent rate enhancement must compare a catalyzed reaction with the appropriate uncatalyzed reaction under specified conditions.[ref]
Kinetics of RNA Degradation by Specific Base Catalysis of Transesterification Involving the 2′-Hydroxyl Group by Yingfu Li and Ronald R. Breaker. Abstract: background cleavage rates and interpretation of catalytic enhancement

Yingfu Li 2026-11-05
Yingfu Li is a biochemist at McMaster University who studies functional nucleic acids, including catalytic DNA and RNA and their use in molecular sensing. His institutional profile and laboratory biography verify the identity and research connection with Ronald R. Breaker.[ref]
Yingfu Li profile at McMaster University. Institutional specialization record; linked laboratory Biography and Research Interests
Li is first author, with Ronald R. Breaker, of the 1999 primary study measuring chemically driven cleavage of RNA phosphodiester bonds. Defined chimeric DNA/RNA substrates allowed the investigators to examine hydroxide-dependent transesterification involving the adjacent -hydroxyl group. This addresses a necessary reference question for studying ribozymes and deoxyribozymes: how rapidly does the corresponding linkage break without the proposed catalyst?[ref]
Kinetics of RNA Degradation by Specific Base Catalysis of Transesterification Involving the 2′-Hydroxyl Group by Yingfu Li and Ronald R. Breaker. Title, byline and Abstract: defined substrates and specific-base cleavage
An original kinetic example illustrates the comparison. Suppose an uncatalyzed linkage has observed rate constant and a tested catalytic condition gives . The rate ratio is . For a simple first-order reaction, the corresponding half-lives are and , approximately 69,315 minutes and 6.93 minutes. These are constructed values, not the study's measured constants. Changing pH, temperature or substrate structure between the two measurements can change the baseline and therefore the meaning of that ratio.
The connection to molecular sensing is that molecular recognition and reaction are distinct functions. A useful signal can depend on binding a target, changing a catalyst's activity and detecting the resulting product. Quantifying each contribution is more informative than observing an output change without identifying its origin.
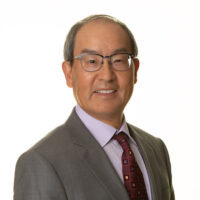
Yingfu Li in the named McMaster University faculty portrait
. The official McMaster engineering faculty page identifies this external photograph as Yingfu Li.