Natural selection involves systematic differences in expected reproductive success associated with variation in phenotype. For a continuing evolutionary response, the relevant variation must be inherited: offspring must tend to preserve the differences being favored. Actual offspring counts also fluctuate by chance, producing genetic drift. Survival matters insofar as it affects contribution to future generations. Genotype fitness is therefore contextual, depending on environment and the life cycle being counted, rather than simply measuring strength or longevity. See Clark, Douglas and Choi, Biology 2e: population evolution.
In chapter IV of his 1859 book, Darwin explained natural selection through preservation of favorable variations and greater chances of survival and reproduction. See Darwin, On the Origin of Species, first edition, chapter IV. The beautiful consequence is cumulative change without foresight: inherited differences are filtered repeatedly by present conditions. Natural selection neither generates a needed mutation on demand nor guarantees progress toward a predetermined goal.
In Charles Darwin's usage, the conditions affecting persistence and reproduction, including interdependence and physical difficulties as well as direct competition.[ref]
On the Origin of Species by Charles Darwin. 1859 edition, chapter III
Selection imposed through human choices about which organisms contribute to later generations. Strong consistent criteria and a controlled environment can produce rapid short-term response while exposing correlated costs.
Selection maintaining more than one inherited variant. Heterozygote advantage and appropriate negative frequency dependence are different mechanisms that can produce this outcome.
Analysis separating selection within groups from selection associated with differences among groups. Group benefit alone does not show that between-group selection overcomes within-group advantage.
Dependence of relative fitness on the frequencies of variants in the population. Its sign and strength must be specified for the ecological context.
Selection in which relative advantage decreases as a variant becomes common, potentially maintaining variation under the stated ecological assumptions.
natural selection in which a variant’s relative fitness increases with its frequency under a specified ecological setting. Shared warning patterns can benefit from prior predator learning.
A framework combining an actor’s effects on its own reproduction with effects on others, weighted by appropriate genetic relatedness and reproductive values. Coefficients and marginal effects depend on the model and population structure.
Selection associated with the indirect reproductive consequences of actions affecting genetically associated recipients. It can favour cooperation without removing all evolutionary conflicts among relatives.
Competition among a restricted set of neighbours or relatives. Benefits to related recipients can be offset when those recipients compete for the same limited breeding opportunities.
A divergence between the outcomes favoured by selection on different individuals, replicating lineages or genetic elements. Conflict can exist without overt fighting.
Conflict among genetic elements whose transmission or expression favours different outcomes despite residence in one organism. Organismal performance alone is not the relevant fitness currency for every element.
Transmission distortion favouring an element over the Mendelian expectation. In a strict usage this acts during meiosis; broader usage also includes biased survival of gametes.
Biased transmission associated with centromere differences during asymmetric meiosis, where only some meiotic products contribute to the next generation.
A modifier reducing a driver’s transmission advantage or harmful consequences. Selection depends on linkage, background and the costs of suppression.
Deviation in inherited allele proportions from the Mendelian expectation. Embryonic viability selection can also distort offspring counts and must be separated from gametic transmission bias.
A genetic element that can spread through a transmission or replication advantage even when it imposes costs on the organism carrying it.
Differences in the outcomes favoured by selection on males and females, for example over mating, fertilization or parental care. Shared benefits from reproduction do not imply identical optima.
A seminal protein studied in Drosophila melanogaster whose transfer affects female physiology and behaviour. Its evolutionary costs and benefits depend on mating regime and measured time horizon.
Conflict mediated by interacting traits encoded at different loci in the sexes, including manipulative traits and resistance.
Different sex-specific optima for a trait influenced by shared genetic variation. Sex-limited expression can reduce the conflict without requiring all genetic effects to become independent.
Reciprocal evolutionary change in traits of the sexes arising through opposed reproductive effects. Correlated morphologies alone need not prove historical reciprocal selection.
Competition among offspring over resources, care or other opportunities. It can interact with parent-offspring conflict by redistributing a fixed supply and altering total parental provisioning.
A decline in the number of surviving offspring within a brood, often associated with limited provisioning. The occurrence of brood reduction alone does not establish an adaptive parental or offspring strategy.
Killing of a sibling, whose ecological and evolutionary explanations depend on resource limitation, asymmetry and the consequences for survivors and parents.
Contingent communication among siblings about their willingness to contest a resource, potentially reducing unnecessary competitive costs.
Differences between parental and offspring strategies favoured by selection, including allocation and duration of care. Costs imposed on other offspring have different weights in the parties’ fitness accounts.
Behaviour or control that reduces the success of selfish actions by other group members. Selection on policing depends on its costs, effects on productivity and genetic or direct benefits to the policing party.
Suppression of worker reproduction by other workers, including discriminatory removal of worker-laid eggs. Genetic incentives and effects on colony productivity can both matter.
Conditional reduction of benefits to a partner that supplies a poor service, potentially changing the returns to exploitation. An immediate physiological response and its evolutionary explanation should be distinguished.
A process by which a heritable change is favoured through an increase in lineage reproductive success under defined conditions. In tumours, mutation opportunity and selection must be analysed separately.
Removal of harmful inherited variants through their lower genotype fitness. Reduced efficacy in small biological populations can permit harmful changes to spread more readily by genetic drift.
Reduction of linked genetic diversity caused by removal of deleterious alleles and their associated backgrounds. It can mimic some genomic diversity patterns attributed to a recent selective sweep.
Opposing effects of the same inherited variant on reproductive performance in the two sexes. Net evolutionary outcomes depend on inheritance, sex-specific expression and the strength of the opposing effects.
Differences in reproductive success arising through access to mates or fertilizations. Conspicuous signals can diverge rapidly under sexual selection without equivalent divergence in the functions required for meiosis.
Behaviour influencing which potential partner contributes to reproduction. The opportunity to choose and the costs of searching constrain its expression.
Differential responsiveness to potential mates or mating cues. Preference must be distinguished from the realized mating pattern produced by encounter, competition and acceptance.
Consider an explicitly idealized haploid population with two inherited types , one allele per individual at the tracked genetic locus, and discrete, nonoverlapping generations. Assume faithful type transmission, no mutation or gene flow, a constant environment, and reproductive contributions independent of type frequency. Let the expected values of offspring surviving to the next census be , with relative genotype fitness .
For frequency , expected offspring contributions are proportional to and . Normalizing gives the deterministic large-population mathematical modelThe denominator is mean relative genotype fitness. For and , . Equivalently, 200 and 800 parents with contribute expected counts 240 and 800. Fractional per-parent expected values are averages, not literal fractional offspring. The ratio of these expectations is a deterministic approximation, not generally the expectation of a random ratio.
The odds multiply particularly simply:Thus : repeated modest advantage can substantially change composition. For and , . The deterministic boundary remains unchanged: natural selection needs existing variation.
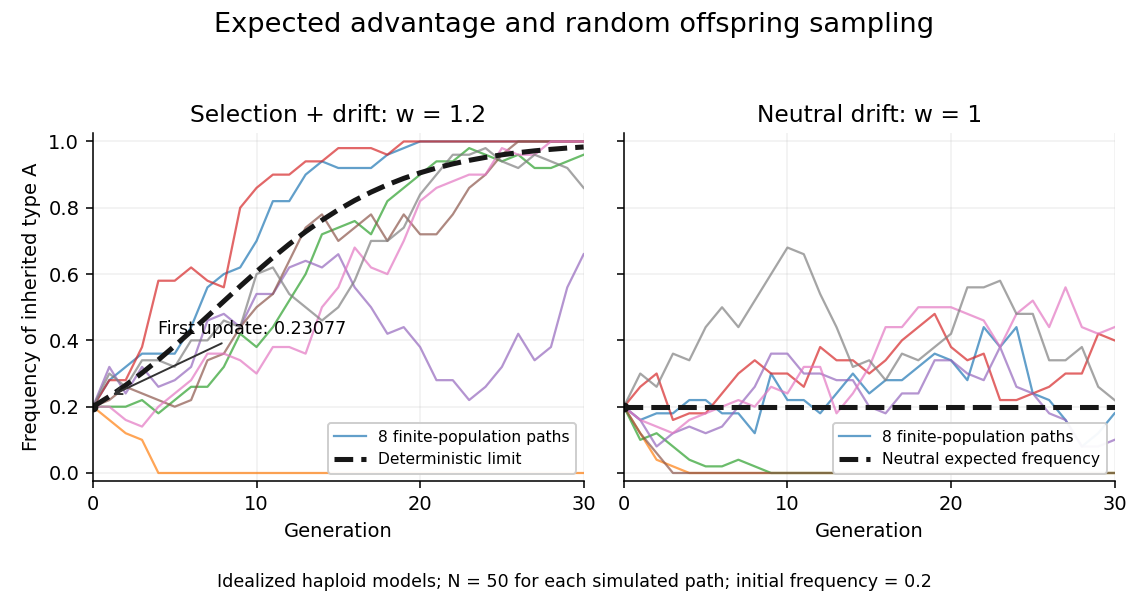
A distinct stochastic extension fixes offspring and samples their types independently using a binomial distribution: , where , then . Its conditional expected value is and conditional variance is . With , the conditional expected value remains , yet realized frequencies wander through genetic drift. With , genetic drift can still lower or lose entirely. Over several generations, the deterministic curve need not equal the mean stochastic trajectory, because the recurrence is nonlinear.
Articles by others on the same topic

Natural selection is a fundamental mechanism of evolution proposed by Charles Darwin. It is the process through which certain traits become more or less common in a population due to differential survival and reproduction of individuals based on their characteristics. Here are the key components of natural selection: 1. **Variation**: Within a population, there is variation in traits (such as size, color, speed, etc.) among individuals. This variation can be due to genetic differences and environmental influences.

