Aerobic respiration uses molecular oxygen as the final electron acceptor. For complete oxidation of glucose, the net material balance isThis records the overall conversion of glucose, molecular oxygen, carbon dioxide and water; it is not one enzyme-catalyzed step, and it omits the separate ATP accounting. For an original stoichiometry check, each side contains six carbon, twelve hydrogen and eighteen oxygen chemical atoms. If exactly of glucose undergoes this complete conversion, the equation requires of molecular oxygen and yields each of carbon dioxide and net water. This is an equation-based calculation, not an observed seed measurement.
The molecular oxygen is reduced to water, rather than being the source of the carbon dioxide's carbon. A formal redox electron balance, using acidic half-reaction notation, makes the roles explicit:Adding and cancelling gives the net equation above. Both half-reactions conserve chemical atoms and electric charge. The Electrons balance a net transfer; they are carried through cellular intermediates, rather than released as a pool of free Electrons. The final respiratory reduction can be written . These equations are bookkeeping, not a tracing experiment that assigns every product oxygen chemical atom to its original molecule.[ref]
Biology 2e by Mary Ann Clark and others. Biology 2e, §7.4, Electron Transport Chain, Figure 7.12: oxygen reduction to water
Glycolysis converts glucose into two pyruvate molecules, with a net two ATP and reduced NADH; it does not directly consume molecular oxygen. Pyruvate processing and the citric acid cycle, also called the TCA cycle, release carbon dioxide and supply reduced carriers. Thus releasing carbon dioxide and consuming molecular oxygen occur at different stages.[ref]
Biology 2e by Mary Ann Clark and others. Biology 2e, §7.2, Outcomes of Glycolysis; §7.3, Breakdown of Pyruvate and Citric Acid Cycle
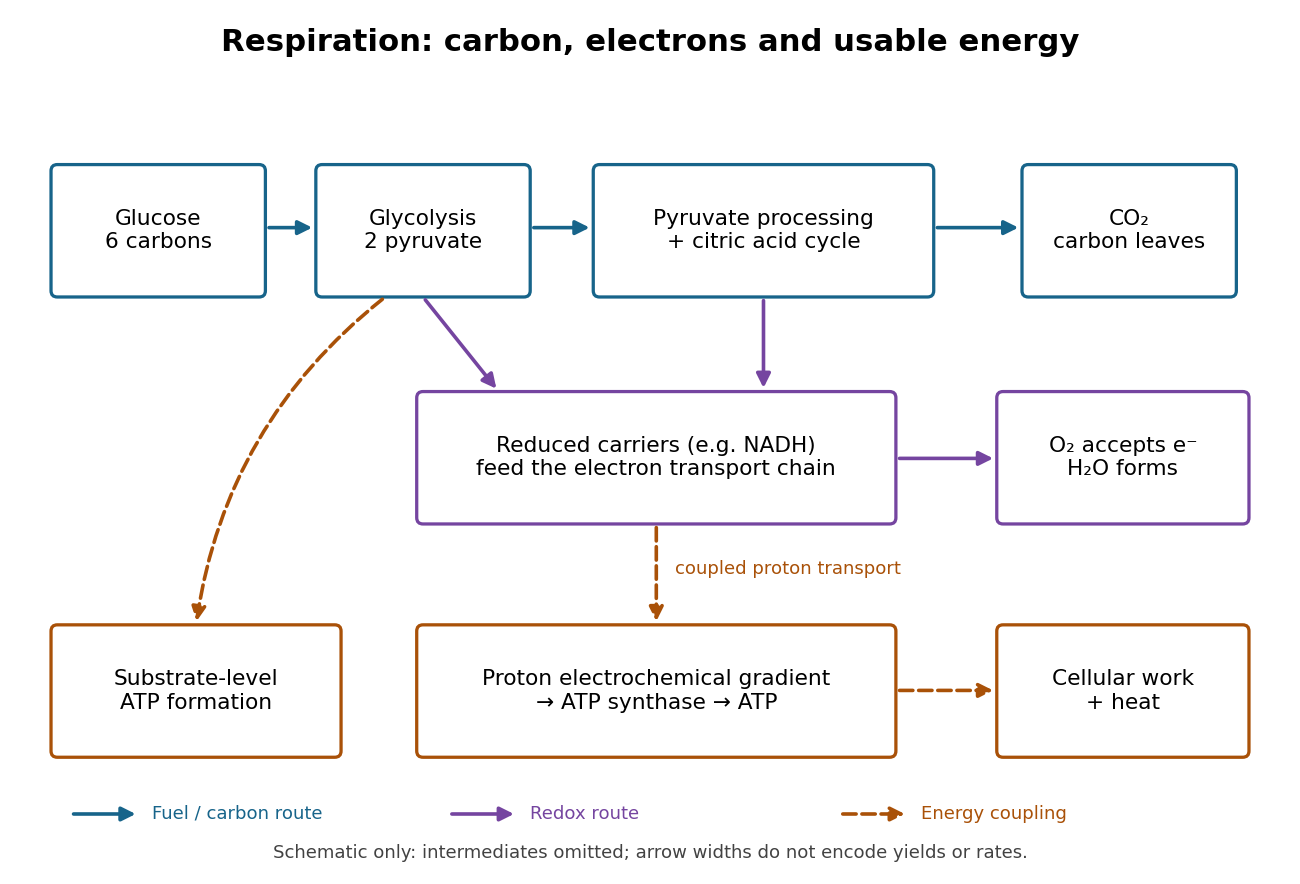

An electron transport chain reoxidizes carriers such as NADH. Coupling some of its redox steps to proton transport establishes an electrochemical gradient; ATP synthase can use that gradient to form ATP from adenosine diphosphate and inorganic phosphate. This is oxidative phosphorylation. A separate route, substrate-level phosphorylation, transfers a phosphate group from a reacting substrate to adenosine diphosphate. In typical eukaryotic biological cells, the respiratory chain occupies the inner membrane of a mitochondrion.[ref]
Biology 2e by Mary Ann Clark and others. Biology 2e, §7.1, Substrate Phosphorylation; §7.4, Electron Transport Chain and Chemiosmosis, Figures 7.12–7.14
The useful achievement is controlled transfer: fuel oxidation can replenish an ATP supply that supports active transport and synthesis. ATP is a reusable chemical carrier, not newly created energy; ATP hydrolysis and the coupled cellular process have their own net free energy balance. Some fuel energy is dissipated as heat.[ref]
Biology 2e by Mary Ann Clark and others. Biology 2e, §7.1, ATP in Living Systems and Energy from ATP; §7.4, ATP Yield
There is no universal yield of or ATP per glucose. Actual ATP recovery depends on carrier transfer routes, coupling and diversion of intermediates to other metabolism. In particular, an oxygen uptake rate cannot be converted into an ATP production rate by assuming one fixed multiplier.[ref]
Biology 2e by Mary Ann Clark and others. Biology 2e, §7.4, ATP Yield: shuttle differences and use of intermediates
Articles by others on the same topic
There are currently no matching articles.