An electron transport chain transfers electrons from an electron donor through electron carriers to a terminal electron acceptor. In the mitochondrial respiratory chain, some transfers drive protons across the inner mitochondrial membrane; their return through ATP synthase can drive ATP formation.[ref]
Molecular Biology of the Cell, 4th edition by Bruce Alberts and others. Chapter 14, Electron-Transport Chains and Their Proton Pumps, Summary: carrier sequence, outward proton transport and ATP synthase
The useful separation is between an electron route and a proton route. The former ends in a redox chemical reaction; the latter changes an electrochemical gradient across a membrane. Energy coupling connects them without making electrons and protons interchangeable. An oxygen readout consequently need not be an ATP readout.
This article focuses on the mitochondrial respiratory chain. Bacteria can use other terminal electron acceptors in anaerobic respiration. In chloroplast light-dependent reactions, light supplies energy and linear electron transport connects water oxidation to NADP+ reduction, releasing oxygen. Thus neither oxygen consumption nor the mitochondrial arrangement defines every electron transport chain.[ref]
Biology 2e by Mary Ann Clark and others. §7.5, Anaerobic Cellular Respiration; §8.2, Generating an Energy Carrier: linear transport from water to NADP+
Transfer of reducing equivalents between a cell and an external acceptor or donor, by direct redox-protein contact, conductive structures or soluble mediators.
An extracellular conductive structure. Composition and conduction mechanisms vary; a filament or pilus image alone does not establish conductivity.
A porin–cytochrome assembly in Shewanella that couples a periplasm-facing multiheme component to an outward-facing cytochrome across the outer membrane.
A copper-containing electron carrier delivering electrons from the cytochrome-b6f pathway to photosystem I in many oxygenic photosynthetic organisms.
Plastoquinone is a mobile lipid-soluble electron carrier in photosynthetic membranes. Its reduction state helps communicate the balance of electron supply and demand between photosystems.
The cytochrome b6f complex transfers electrons between the two photosystems in oxygenic photosynthesis and contributes to proton-gradient formation. Its regulated throughput links lumen conditions to intersystem electron flow.
NADH supplies two electrons to respiratory complex I, then ubiquinone, respiratory complex III, cytochrome c and cytochrome c oxidase; terminal oxygen reduction forms water. Succinate dehydrogenase, or respiratory complex II, supplies another entry to ubiquinone. Respiratory complex I, respiratory complex III and cytochrome c oxidase move protons outward; respiratory complex II does not.[ref]
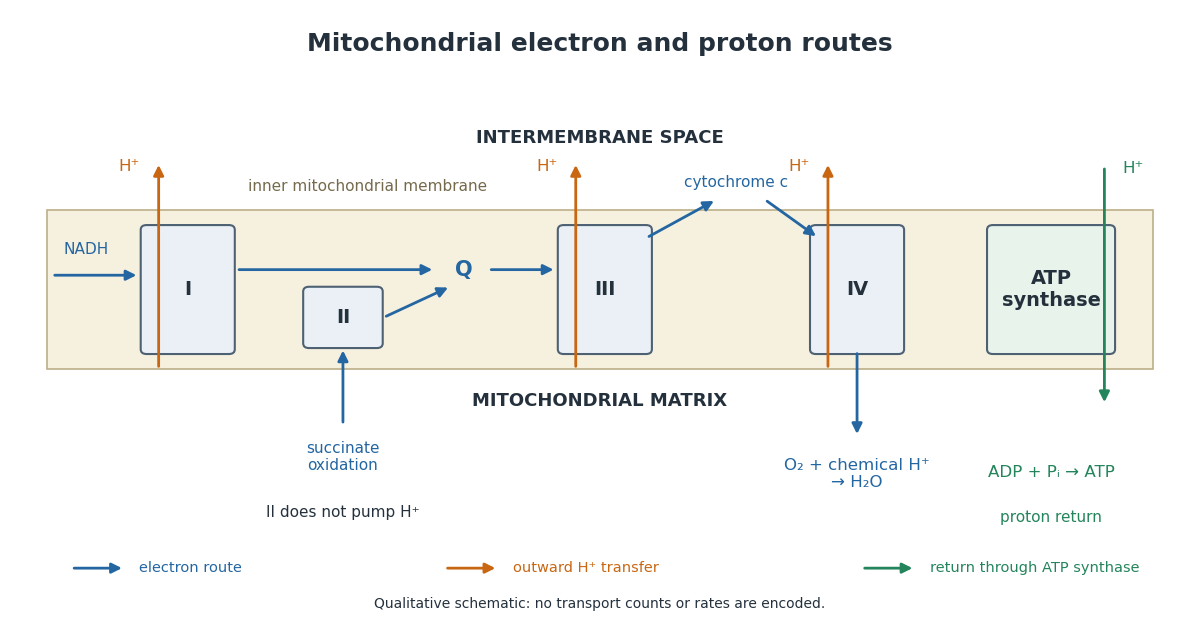
For an original electron balance, supply exactly of NADH to an ideal preparation with no other electron donor or competing electron acceptor. The donor supplies of electrons. Complete reduction of one oxygen molecule needs four electrons, so the corresponding oxygen consumption is . Adding the two formal half-reactions makes the result explicit:The cancelling electrons determine the donor-to-oxygen ratio. These chemical equations do not count transmembrane protons or determine an ATP yield. Chemical protons consumed in water formation and transported protons have different roles in the ledger.
An electron carrier cycles between oxidation and reduction. Ubiquinone carries two electrons, while cytochrome c carries one at a time.[ref]
Biology 2e by Mary Ann Clark and others. §7.4, Q and Complex II; Complex III: mobile carriers and electron capacities
For example, transferring the two electrons supplied by one NADH requires two one-electron deliveries by cytochrome c. It does not require two permanently consumed cytochrome c molecules: an available electron carrier can unload, return and reload. Electron carriers recycle material while the net redox conversion supplies free energy.
Respiratory control links mitochondrial oxygen consumption to demand for ATP. When ADP permits faster ATP synthase turnover, proton return lowers the opposing electrochemical gradient, permitting faster electron transport.[ref]
Molecular Biology of the Cell, 4th edition by Bruce Alberts and others. Chapter 14, Electron-Transport Chains and Their Proton Pumps, Respiratory Control Normally Restrains Electron Flow Through the Chain
The mitochondrial oxygen electrode assay tests this connection by changing ADP availability while observing oxygen. A slowed reaction rate alone cannot locate the cause: depleted substrate, scarce oxygen, impaired enzymes and a strong opposing electrochemical gradient can all restrict turnover. A renewed response to ADP helps distinguish these possibilities.
In Respiratory enzymes in oxidative phosphorylation. I. Kinetics of oxygen utilization (1955), Britton Chance and G. R. Williams examined isolated liver mitochondria in isotonic medium with substrate and inorganic phosphate. A one-millilitre optical cuvette held the suspension. A vibrating platinum electrode lay outside the light path; calibrated electric current followed dissolved oxygen, with rapid changes recorded by a galvanometer oscillograph. Air-saturated and oxygen-depleted readings checked sensitivity. Their Figure 2 shows ADP additions accelerating oxygen consumption, followed by return to slow respiration; repeated additions restored acceleration. Figure 4B compares delayed substrate addition after ADP incubation with the reverse order, supporting little unrelated ADP loss in that preparation. These comparisons support coupling to ADP utilization. The authors discuss dilution, sensitivity changes and atmospheric oxygen entry, which especially biases slow respiration. The readout did not directly measure the membrane potential or prove the later chemiosmosis mechanism.[ref]
Respiratory enzymes in oxidative phosphorylation. I. Kinetics of oxygen utilization by Britton Chance and G. R. Williams. pp. 383–386, Preparations and Method, Figures 1–2; pp. 387–389, Endogenous Substrate and Figure 4B; Figure 5: rapid recording
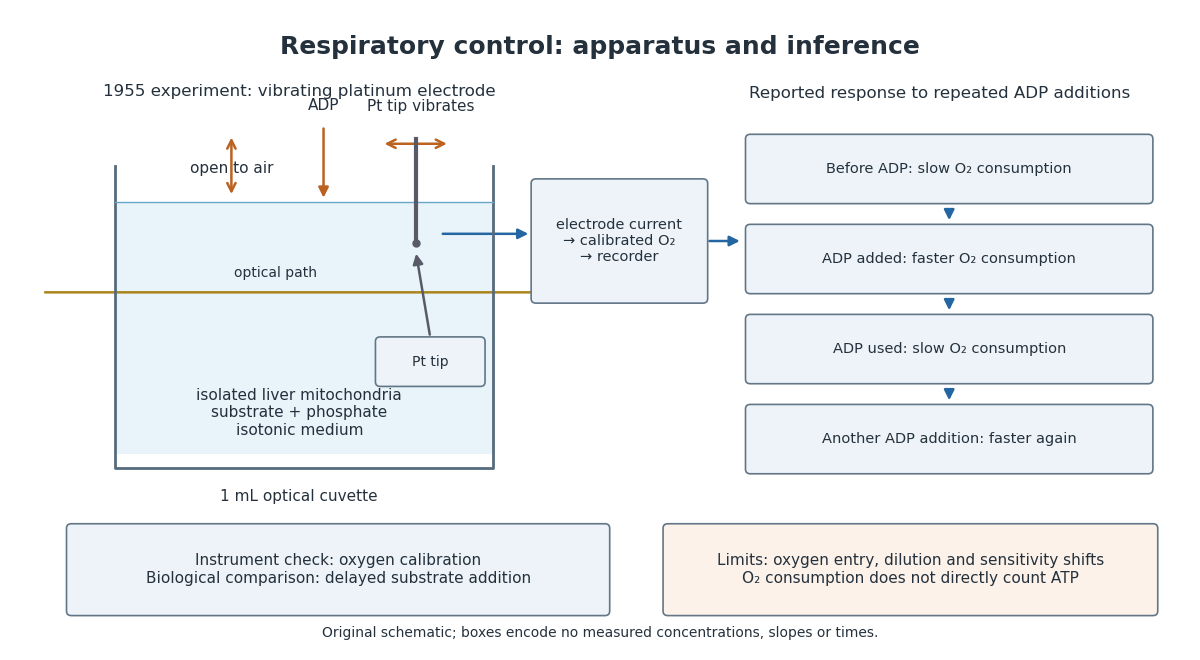
A control can test either the instrument or the biology. Calibrating electric current against oxygen checks the former; comparing responses before and after an ADP addition checks the latter. A valid calibration cannot by itself establish ATP formation, and a repeatable biological response cannot by itself fix an instrument's sensitivity.
The respiratory control ratio divides the oxygen consumption rate during ADP-stimulated respiration by that after supplied ADP has been used. It compares reaction rates, not ATP formed per oxygen.[ref]
Respiratory enzymes in oxidative phosphorylation. I. Kinetics of oxygen utilization by Britton Chance and G. R. Williams. pp. 386–387, Figure 2 and discussion of the ratio of respiration rates with and without ADP
A large ratio means strong stimulation under the comparison's conditions; it is not a universal measure of all mitochondrial functions.
For a constructed example, choose constant suspension volume and oxygen concentration declines of and during the two comparison windows. Assume no gas exchange or dilution and a correctly calibrated readout. A derivative converts each concentration slope into an amount of substance consumption rate:The common volume cancels in the ratio, so dividing the positive slope magnitudes gives the same answer. These are chosen inputs, not the 1955 observations. If an uncorrected influx of of oxygen occurred in both windows, the apparent rates would instead be and , giving . The same absolute error can inflate a ratio because it removes a larger fraction of its smaller denominator.
Articles by others on the same topic



Good animation explaining it: Video "Electron transport chain by HarvardX (2017)".