For this concave recruitment map, the extinction state is invariant because . Near extinction, with multiplier above one, so small positive populations initially grow. The strict concavity means marginal recruitment decreases as population increases. More precisely, for ,since . Thus per-capita recruitment decreases and the graph bends downwards from an initial slope greater than that of the identity line.
A positive fixed point, if present, is the unique positive intersection with : the strictly decreasing ratio can cross one at most once. The sketch shows the usual saturating example , which crosses at .
The three assumptions alone do not guarantee this crossing. For example satisfies all three and remains strictly above for every . An extra large-population restriction, such as somewhere, supplies existence. Keeping this distinction avoids inventing a carrying capacity that is not implied by the printed hypotheses.
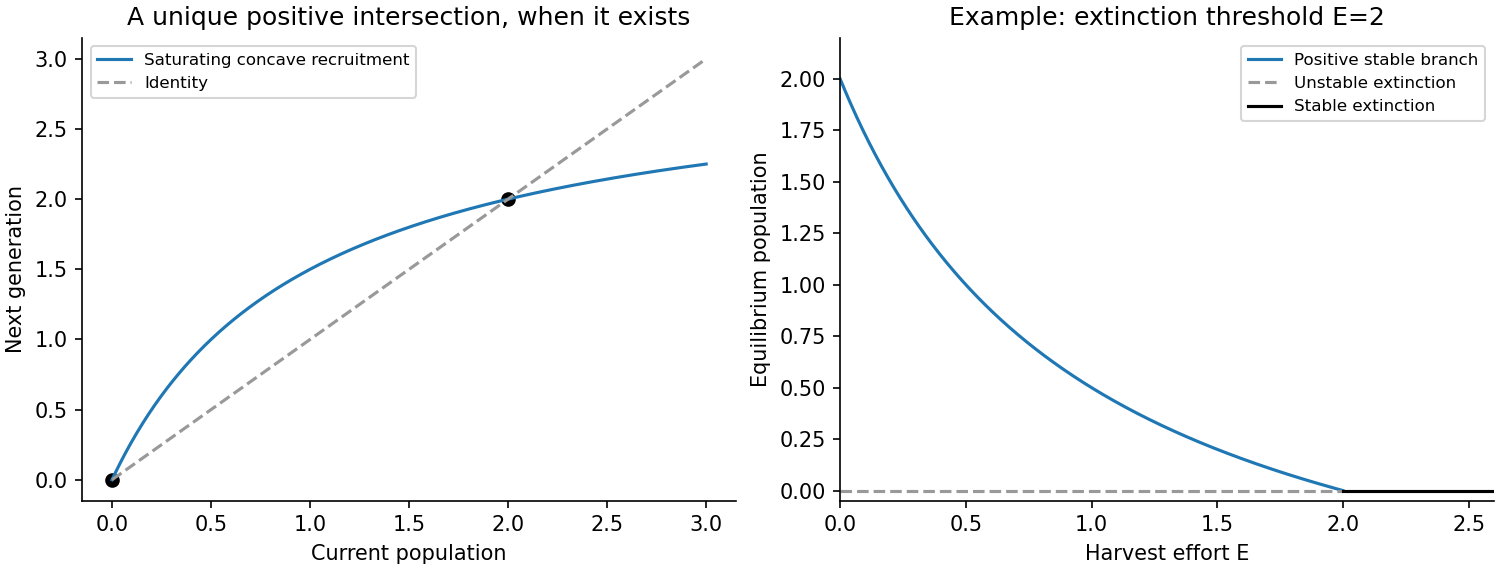
Concave recruitment and the identity line, with loss of the positive equilibrium under harvesting
. Details. Let be a fixed point and put . Taylor expansion gives , so the linear perturbation is . Thereforeis the condition for linear asymptotic stability. A multiplier in gives monotone decay; one in gives alternating decay. If its magnitude exceeds one, perturbations grow. Magnitude one is nonhyperbolic and needs nonlinear analysis.
Strict concavity and already give . Thus the remaining stability requirement is . If is additionally nonnegative on the entire half-line, strict concavity prevents its derivative becoming negative there, since it would then force eventually negative. Under that stronger global population-map assumption the positive fixed point is automatically stable. The printed local slope and concavity information, without that global nonnegativity requirement, does not by itself rule out a flip instability.
With constant-effort harvesting, the constant-effort model isThe extinction multiplier becomes , so extinction is linearly stable when . At its multiplier crosses . Values large enough to make the next population negative lie outside the physical validity of this untruncated harvest model.
Any positive fixed point solves . Since that ratio is strictly decreasing, there is at most one such point, and it decreases with effort. Differentiating the fixed-point equation yieldsIf the unharvested positive branch exists, it continues for and approaches zero as . This follows because its required ratio lies between and ; its intersection lies between zero and the unharvested fixed point. There is no positive fixed point for .
The positive-state multiplier is by concavity. It is stable precisely whenCrossing can change stability through a flip, but the direction of change is not fixed by the three assumptions: has no prescribed sign. In the illustrated saturating example, increasing effort eventually removes the positive branch at extinction. The finite upper stability bound for the algebraic extinction map should not be interpreted as a physically meaningful recovery of a population at unrealistically large harvest effort.
A steady population is a root . To linearize one needs differentiable near that root, an extra local regularity assumption beyond the source's continuity. Setting gives , hence at linear order.
Thus gives linear asymptotic stability and gives instability. If , linearization is inconclusive. In a one-dimensional phase line, the more general nonlinear test is whether the vector field points towards the root from both sides. At the physical boundary , only the right-hand side matters. Continuity alone does not guarantee uniqueness of trajectories, so a standard well-defined flow also presumes a local uniqueness condition, such as local Lipschitz continuity.
The four nonnegative equilibria are . Since all factors are positive below , the sign of on consecutive intervals isThe phase line therefore points away from zero, towards , away from , and towards . Equivalently , and at each simple positive root , . Their signs alternate negative, positive, negative.
Hence extinction and are unstable, while and are asymptotically stable. Initial positive populations below tend to ; those above tend to ; an initial population exactly at remains there. This is bistability with a threshold separating the two basins.
Put . The harvested vector field is . Define the extinction threshold , and let be the positive local maximum of , with . Writing , givesPositive equilibria are intersections of with the horizontal line . A lower stable branch in exists exactly for . A pair in exists exactly for : its smaller member has and is unstable; its larger member has and is stable. At a positive root the linear eigenvalue is , which proves these claims. Extinction has eigenvalue , becoming stable for .
The harvested bistable population thresholds determine the behaviour. If , the upper stable population and its unstable separator first disappear in a saddle-node bifurcation. Populations then tend to the remaining lower stable state until that branch reaches extinction at ; beyond it extinction attracts every positive initial state. If , the lower stable branch reaches extinction first. For , extinction and the upper positive state are both stable, separated by the middle unstable root. Increasing effort through then destroys the remaining positive attractor, causing a sudden collapse to extinction. If , both events occur at the same effort at different populations.
At , near zero the leading term is , so extinction attracts from the physical right side algebraically, despite its zero linear eigenvalue. At , the double positive root is semistable: locally , attracting from above and repelling from below. These critical cases matter for exact initial data. The figure shows examples of both strict threshold orderings.
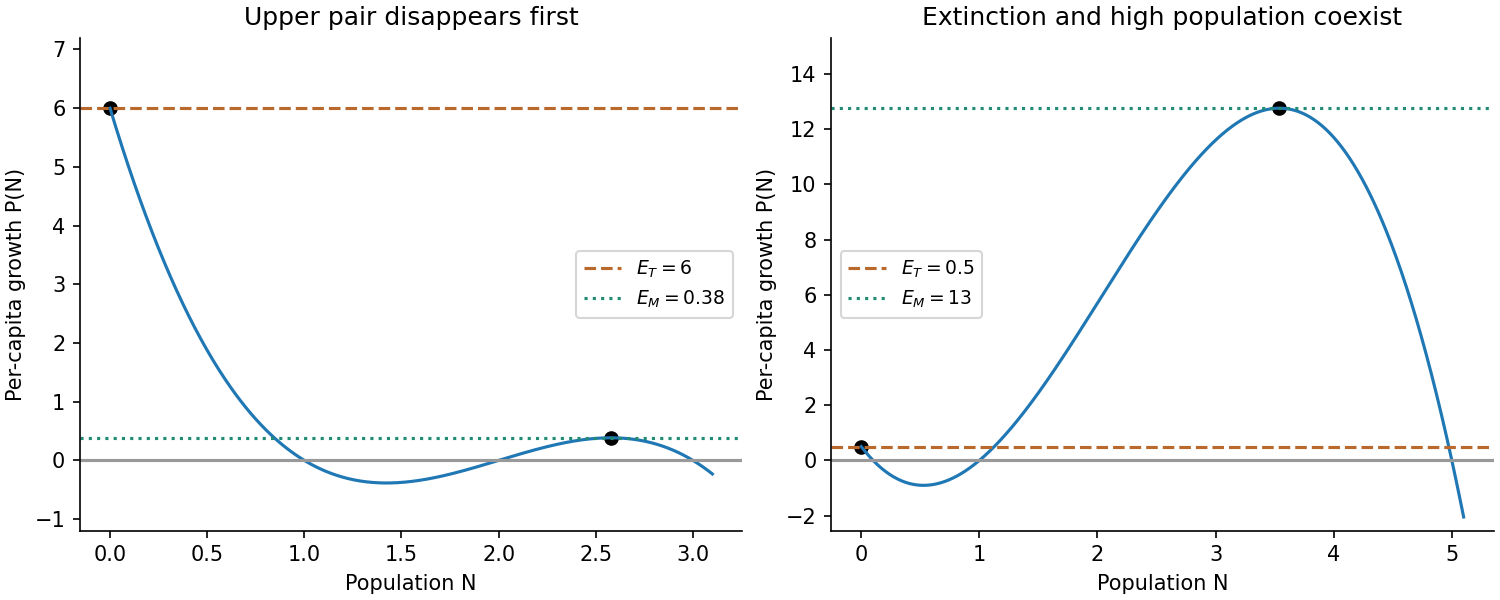
Two possible orderings of the extinction and saddle-node harvesting thresholds
. Details. The law of mass action makes each elementary reaction rate proportional to the product of its reactant concentrations, with the stoichiometric change determining its contribution. Let be maintained constant, and let be the diffusion coefficients. The first reaction consumes two molecules, the second creates one net , the third consumes one each of , and the fourth consumes while creating . Fick's laws for diffusion giveHere the standard deterministic convention takes the event rate of the first reaction as , so its loss is . A convention absorbing a combinatorial factor into leads to the same nondimensional model after consistently redefining that rate constant. The maintained reactant makes this an open chemical model; there is no conservation law requiring to decrease with reaction progress.
Choose , , , and an independently selected positive representing its reference or supplied concentration. Set , , , . Dividing the first equation by and the second by yields the stated system withThe parameter can be changed through the chosen or physically supplied reference concentration while these other combinations remain fixed. The combinations satisfy for this reaction mechanism, so they need not be algebraically independent. The spatial scale makes the diffusion coefficient one, and the time and scales balance linear autocatalytic growth against the quadratic loss.
The equal-diffusivity Fisher reduction uses equal diffusion coefficients and the invariant relation . The second equation then requires , while the first becomes . They agree whenThis reduction requires compatible initial and boundary data on that invariant relation. Tuning a parameter alone does not force arbitrary solutions of the two-field system onto it. For positive physical , the displayed normalization also requires . More generally the line works when ; the same positivity restriction remains for .
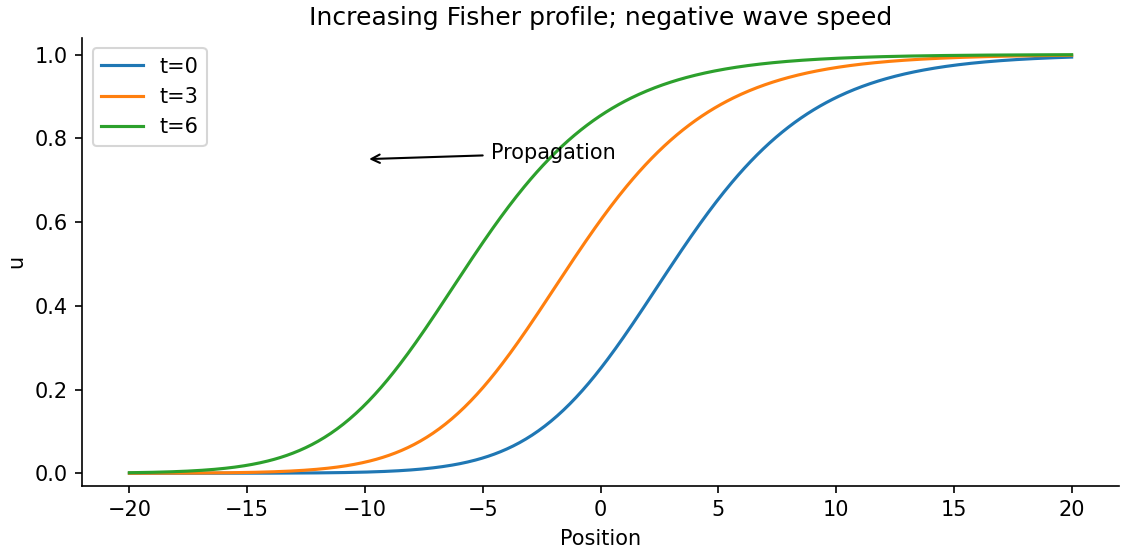
Let and with , . The profile equation is . Multiplication by and integration givesConsequently : the increasing front moves left, with the state invading . Linearization at its leading edge gives real monotone exponents only when , yielding the usual Fisher front speed range. A convenient exact example isSubstitution verifies it and the figure shows its leftward displacement. The source uses for the end limits after defining ; they denote the same spatial coordinate here.


Yes. An immobile concentration can still change locally through reaction while diffusing transports activation. Vanishing diffusion of one component does not prohibit a propagating reaction front.
In the invariant special case , the first equation is already Fisher's equation with growth coefficient one, so it has travelling fronts regardless of . A one-diffuser reaction front also gives a coupled example with nonzero . For , the equations with areFor , choose , , and setIndeed and , giving the second equation. In the first, division by leaves , whose constant and coefficients both vanish with these choices. Ahead of the left-moving wave ; behind it . This explicitly demonstrates a travelling front with substrate depletion but no diffusion, rather than relying solely on the uncoupled special case.
A uniform steady state satisfies . Set , and keep only first-order terms in the perturbations. Since the base state is constant, its Laplacian vanishes. Taylor expansion givesThe zero-flux boundary conditions linearize to homogeneous Neumann conditions, . The off-diagonal entries of the Jacobian describe the cross-effects of the two chemicals, while the diagonal entries describe local self-response.
A diffusion-driven instability means that the homogeneous reaction equilibrium is asymptotically stable against spatially uniform perturbations, but adding diffusion makes at least one admissible spatially nonuniform mode grow. Thus the eigenvalues of must have negative real parts, while has an eigenvalue with positive real part for some positive Neumann Laplacian eigenvalue on the actual domain.
The instability is driven by different diffusion responses acting together with reaction feedback. It is not merely an equilibrium that was already unstable without diffusion. On a bounded domain the permitted wave numbers are discrete, so an algebraically unstable continuous band must also contain an actual spatial eigenmode.
Write , , , , . Stability without diffusion requires and . For a mode with , the characteristic equation isFor positive diffusivities the trace stays negative for every , so growth can occur only if . Put . This upward-opening quadratic has a negative interval at positive exactly when and , orIf , the right side is , impossible. Equivalently diffusion would merely subtract from both reaction eigenvalues. Thus unequal diffusivities are necessary.
The potentially unstable band has endpointsThese are necessary continuous-wave-number conditions. Actual instability on the specified bounded domain additionally requires an allowed strictly between them. The strict inequalities exclude neutral onset and presume both diffusivities are positive, as in an ordinary two-chemical diffusion model.
After relabelling the chemicals if necessary, take and . At least one diagonal entry must be positive because , whereas their sum is negative. Since their product is negative and , the off-diagonal product must be negative and sufficiently large in magnitude. The two possibilities areIn the first, activates its own production and stimulates , while suppresses : an activator-inhibitor mechanism. In the substrate-depletion pattern mechanism, promotes the autocatalytic species , which consumes or suppresses : a substrate-depletion mechanism. These are different biological interaction signs, not merely two drawings of the same feedback. Suitable relative magnitudes and sufficiently different diffusivities are still required; the sign pattern alone does not guarantee a Turing instability.
For Neumann boundaries the correct eigenfunctions include zero indices:Their squared wave number is . The constant pair is reaction-stable. Instability requires , using the band derived above. If both side lengths are large, the wave-number spacings are small enough that admissible modes can enter the band in either direction, including mixed modes. This does not mean the single mode necessarily stays unstable as lengths tend to infinity: its wave number eventually tends to zero below the band. Rather, increasingly fine wave-number spacing permits some suitable higher integers.
Thin-domain Turing mode selection applies if , every mode with has and is stable. A sufficiently large can nevertheless admit an integer with and . HenceThe printed range starting both indices at one excludes these purely longitudinal modes and cannot imply the requested conclusion. It also omits the constant mode. Further, each allowed spatial eigenfunction generally has two temporal eigenvalue branches of , with coefficients along their eigenvectors; a single unrestricted scalar is shorthand for those branches rather than a complete general expansion.
Domain geometry can select biological pattern dimension even when the same reaction parameters and diffusion coefficients are used. A sufficiently wide developing tissue can admit instabilities with variation in two spatial directions; nonlinear development may produce spots, labyrinths or other two-dimensional patterns. A thin strip suppresses transverse unstable modes, allowing primarily bands whose concentration varies along its long axis and is nearly uniform across its width.
This is a mechanism for shape-dependent pattern selection during growth: increasing tissue width can admit additional transverse modes without changing the local chemical interactions. Linear instability predicts initial wavelengths and permitted directions, not the eventual stable spot or stripe pattern; nonlinear saturation and boundary geometry determine that later outcome. Zero-flux boundaries also mean these modes arise through internal redistribution and reaction rather than externally prescribed chemical concentrations.
Articles by others on the same topic
There are currently no matching articles.