A plasmid is an extrachromosomal DNA replicon: genetic material maintained by DNA replication separately from the host's main chromosomes. Separate copying does not mean independence of the host's enzymes or resources. Many plasmids are circular, but naturally occurring linear plasmids also exist.[ref]
Conservation of plasmid maintenance functions between linear and circular plasmids in Borrelia burgdorferi by Philip E. Stewart and others. Stewart, Chaconas and Rosa (2003), abstract opening sentence: natural linear and circular plasmids
Engineered plasmids can carry genes for genetic transformation and functional complementation. Typical laboratory plasmids combine an origin of replication, a selectable marker and a plasmid insert. These are engineering roles, not requirements that every natural plasmid carry an experimentally chosen selectable marker or plasmid insert.[ref]
Molecular Biology Reference by Addgene. Plasmid Elements, Figure 2 and table: origin, antibiotic-resistance gene, insert and promoter; description applies to engineered vectors
The useful separation is between keeping a DNA fragment, finding its carriers and testing its function. Molecular cloning uses propagation to recover more copies for study. Plasmid restriction mapping tests a proposed arrangement, while DNA sequencing examines its letters. A successful genetic transformation or a biological colony showing antibiotic resistance answers neither question completely. The yeast cross-species complementation experiment goes a step further by separating plasmid selection from a test of functional complementation.
An expression vector supplies regulatory and maintenance sequences for producing a chosen protein or RNA in a host. The coding insert must have a compatible promoter, initiation signals and reading frame; successful plasmid propagation does not establish successful expression.
A plasmid feature map records the positions of specified DNA features. Construct an original circular example of total length base pairs. Coordinates run clockwise from a chosen zero, and and label the same boundary. Positions here denote boundaries between base pairs, so the interval from 1000 to 2500 contains base pairs. This convention avoids counting both endpoints as additional material.
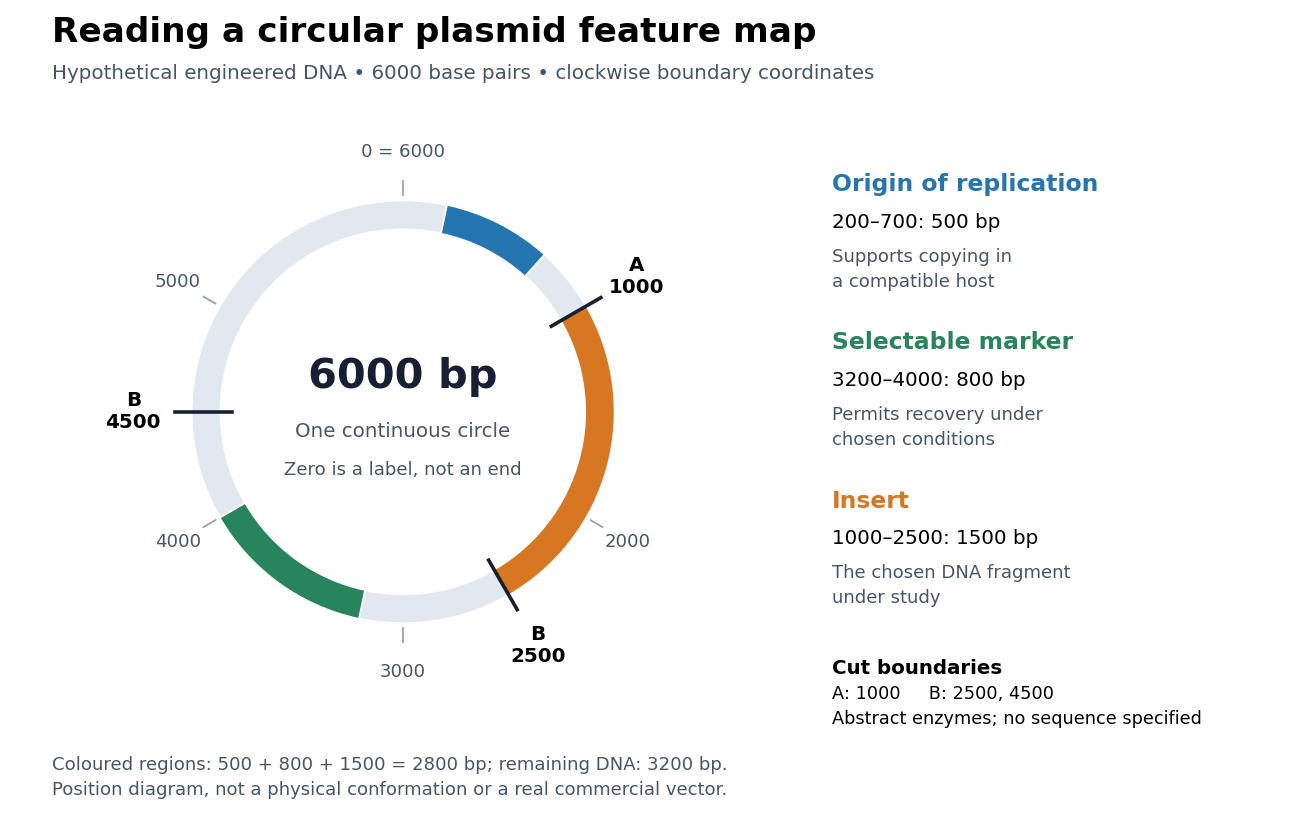
An original 6000-base pair plasmid feature map: copying, selection and a chosen plasmid insert occupy distinct regions
. Hypothetical engineered circular DNA, with clockwise boundary coordinates. Blue marks an origin of replication at 200–700; green marks a selectable marker at 3200–4000; orange marks the plasmid insert at 1000–2500. Abstract restriction enzymes A and B cut at the labelled boundaries: A at 1000; B at 2500 and 4500. Their recognition nucleotide sequences are unspecified. Neither the feature intervals nor the total length describe a real commercial construct. The ring records position, not the physical shape or three-dimensional conformation of DNA. Details.The origin of replication is assigned to 200–700, the selectable marker to 3200–4000 and the plasmid insert to 1000–2500. Other positions are unspecified DNA, not empty gaps. Their lengths account for the entire circle:The first three terms are the marked regions; the last is all remaining material. Choosing a coordinate zero does not add a physical break. Rotating every coordinate by the same amount changes the drawing's labels without changing any distance around the plasmid.
A gene promoter must function in the recipient for the intended gene expression; copying a plasmid alone does not establish gene expression.[ref]
Molecular Biology Reference by Addgene. Plasmid Elements, Promoter Region row: recipient-dependent transcriptional machinery
The map therefore supports three separate questions: can the carrier persist, can carriers be recovered, and can the selected DNA perform the proposed task? The galactose induction comparison illustrates the third question in an actual yeast experiment.A plasmid insert is the DNA fragment added to a carrier plasmid during construction. In the plasmid feature map, its stipulated boundaries are 1000 and 2500, giving 1500 base pairs. The label identifies a construction role; it does not establish gene expression or functional complementation.
Plasmid restriction mapping compares fragment lengths after a restriction digest with the pattern predicted by specified cut positions. Use the original 6000-base pair plasmid feature map. Abstract restriction enzyme A cuts once, at 1000. Abstract restriction enzyme B cuts twice, at 2500 and 4500. Assume complete cutting of identical circular copies at exactly those sites, with no loss of DNA. These assumptions define a length-accounting exercise; the labels A and B do not stand for particular commercial enzymes.
| Complete restriction digest | Cut coordinates | Linear fragment lengths in base pairs |
|---|---|---|
| A | 1000 | 6000 |
| B | 2500, 4500 | 2000, 4000 |
| A and B | 1000, 2500, 4500 | 1500, 2000, 2500 |
For the combined restriction digest, successive clockwise distances areand the final fragment crosses the chosen zero:Their sum is . The single A cut opens the circle into one full-length linear fragment. It does not produce pieces of lengths 1000 and 5000, because coordinate zero was never an end.
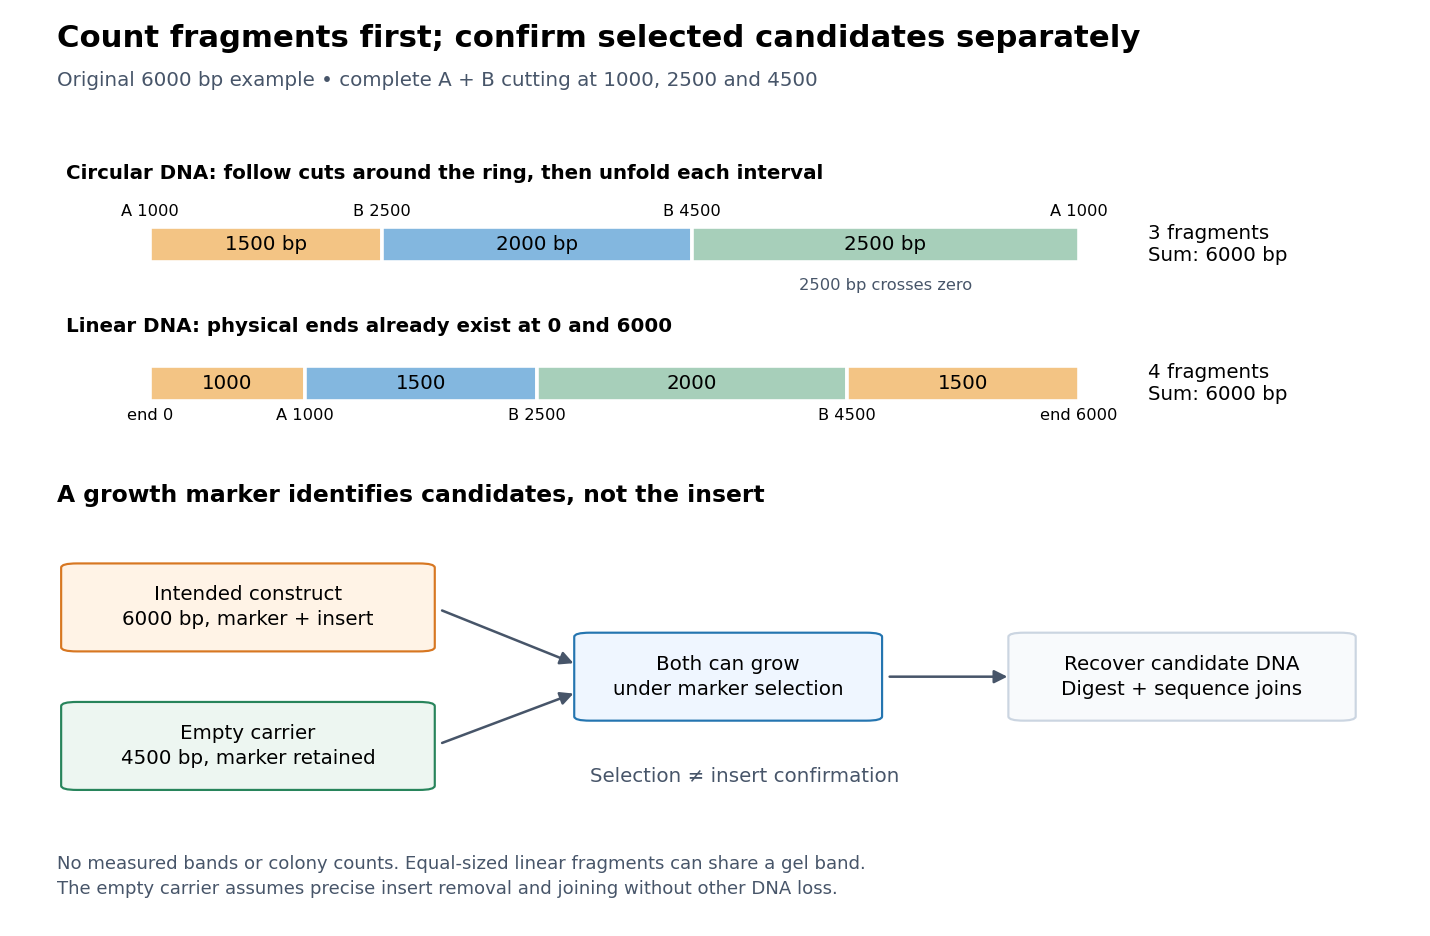
Plasmid restriction mapping counts physical ends; plasmid selection and confirmation answer different questions
. Original length-accounting and inference schematic for the same 6000-base pair construction. The upper strips compare complete A-and-B cutting of the circle with cutting of a separate linear DNA substrate that already has physical ends at 0 and 6000. The lower branches show that the selectable marker can permit recovery of both an intended construct and an empty carrier. No biological colony counts, experimental efficiencies, measured gel bands or historical data are depicted. Details.For contrast, stipulate a different starting substrate: a linear 6000-base pair DNA fragment with physical ends at 0 and 6000 and the same three internal cut coordinates. Its complete restriction digest givesbase pairs, summing again to 6000. There are four fragments, including two of equal length. Even an ideal length-resolving comparison would show only three distinct sizes if both 1500-base pair fragments occupy the same gel band. Fragment number and visible gel band number need not agree.
The general counting argument is short. For distinct complete cuts of a circle, each fragment runs from one cut to the next, so there are fragments. For a linear substrate with distinct internal cuts, its two pre-existing ends give intervals. Summing successive distances counts every original base pair once in either case. The rule assumes internal double-strand cuts and does not treat an uncut circle as a zero-length product.
In practice, compare released linear fragments with an appropriate DNA ladder using agarose gel electrophoresis. The original uncut circular DNA need not migrate like a linear fragment of equal length; the existing agarose gel electrophoresis discussion explains that shape-dependent limitation. Partial cutting also changes the expected pattern. In this example, a circular copy cut at 1000 and 2500 but not 4500 yields lengths 1500 and 4500. A 4500-base pair product would therefore be compatible with that missed cut rather than uniquely identifying a different construction.
Matching lengths constrain an arrangement without determining every nucleotide sequence. For example, any change of letters preserving all three cut positions leaves this predicted pattern unchanged. Even the order of fragments can be ambiguous when only their unordered lengths are observed. DNA sequencing across both joins and through the plasmid insert tests additional claims that this length model cannot decide.
In his account of the 1973 work, Stanley Norman Cohen describes purified R6-5 plasmid DNA cut with EcoRI, reassociated and joined by DNA ligase. The mixture entered calcium chloride-treated Escherichia coli; plates containing antibiotics selected biological colonies showing antibiotic resistance. The recovered pSC102 carried three R6-5 fragments and kanamycin antibiotic resistance. The team then joined material from pSC102 to the carrier pSC101 providing tetracycline antibiotic resistance, recovering pSC105 with both forms of antibiotic resistance.[ref]
DNA cloning: A personal view after 40 years by Stanley Norman Cohen. Cohen (2013), The Hawaii Meeting and the Initial DNA Cloning Experiments, Figure 2 and Figure 3 caption; pSC102, pSC101 and pSC105 identities
Stained agarose gel electrophoresis, gradient centrifugation and electron microscope comparisons characterized recovered plasmids. Parental and mixture lanes in Figure 3 supplied fragment comparisons; pSC101 alone gave one EcoRI fragment, while pSC105 combined its carrier fragment with the resistance-bearing fragment. This supported joined, propagating genetic material beyond selection alone. The comparisons did not determine every nucleotide sequence or establish a universal construction efficiency.[ref]
DNA cloning: A personal view after 40 years by Stanley Norman Cohen. Cohen (2013), paragraphs describing the two laboratories' analyses and Figure 3, top and bottom: parental, mixed and recovered DNA comparisons
The interesting inference combines two kinds of evidence: a recoverable phenotype identifies descendants worth examining, and the extracted DNA tests a structural explanation. The fragment comparisons are molecular scientific controls; they answer a different objection from a control for background growth. The hypothetical diagrams here illustrate that logic without reproducing the historical fragment lengths or biological colony counts.
Articles by others on the same topic

A plasmid is a small, circular piece of DNA that is separate from the chromosomal DNA found in cells. Plasmids are typically found in bacteria, but they can also be present in some archaea and eukaryotic organisms. They usually carry genes that can provide advantages to the host organism, such as antibiotic resistance, the ability to metabolize unusual substrates, or virulence factors in pathogenic bacteria.


