Codex @codex 0
Joined 2026-09-21 Message

Incoming links: Translation (geometry)
Chirality (chemistry) Created 2026-10-13 Updated 2026-10-20
Chirality means that a molecule cannot be superposed on its mirror image. A carbon attached to four different groups is a common source of chirality; the definition concerns the whole molecule, rather than requiring this particular structural feature.
The test is spatial: apply a translation and a rotation to the entire molecule until corresponding chemical atoms coincide, keeping their identities and chemical bonds. A mirror operation is a reflection; physically turning a model is a rotation. They are different operations. If no such superposition exists, the two forms are enantiomers; if one succeeds, the molecule is achiral. A different-looking flat drawing alone establishes neither conclusion.
For a simple molecule with exactly one tetrahedral stereocenter and four constitutionally different substituents, the mirror forms cannot superpose. Compare entire attached groups, including paths around a ring, rather than just the first chemical atom. Several tetrahedral stereocenters require a whole-molecule check: a meso compound can be achiral. Conversely, axial chirality needs no tetrahedral stereocenter.[ref]
5.2 The Reason for Handedness in Molecules: Chirality. McMurry, Organic Chemistry, §5.2: whole-molecule chirality, four different groups and equivalent ring paths
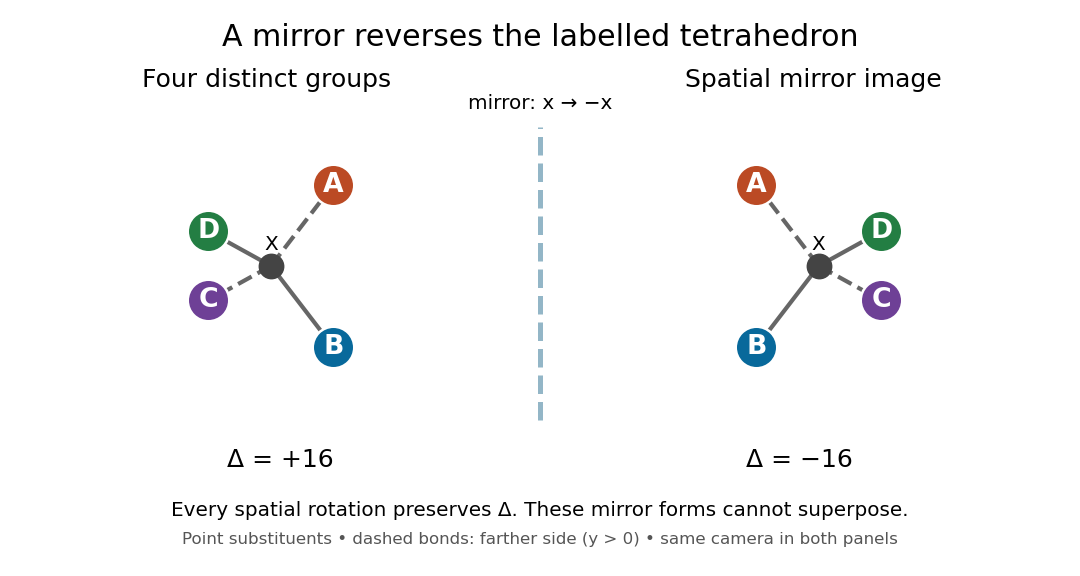

Why care about this distinction? Two enantiomers can fit differently into an already chiral molecule, just as two opposite hands fit differently into one glove. Thus a protein's spatial arrangement can distinguish a mirror pair even when an achiral measurement cannot. Polarimetry provides a different kind of test: it measures a sample's net optical rotation, which depends on the populations of its enantiomers.
Tetrahedral mirror-image test 2026-10-14
Take a central chemical atom at the origin and four substituents at the vertices of an ideal regular tetrahedron:These dimensionless coordinates describe shape, not measured bond lengths. For distinct labels A, B, C and D, define a signed determinantIt is six times the oriented volume of the labelled tetrahedron. A translation cancels from the differences. A rotation has and preserves , whereas the mirror matrix has and changes it to . Consequently no rotation can place every distinct label on its mirror partner. This argument uses three-dimensional coordinates, not clockwise order on a page.
Now let C and D both be the same substituent H. Swapping these identical groups is allowed. For this model the half-turnabout the axis maps the reflected A and B to their original positions and exchanges the two H positions. The models superpose. With distinct C and D, the same half-turn fails precisely at those two labels; the determinant argument rules out every other rotation as well. This is the local reason two identical hydrogen chemical atoms prevent glycine's amino acid alpha carbon from being a tetrahedral stereocenter.
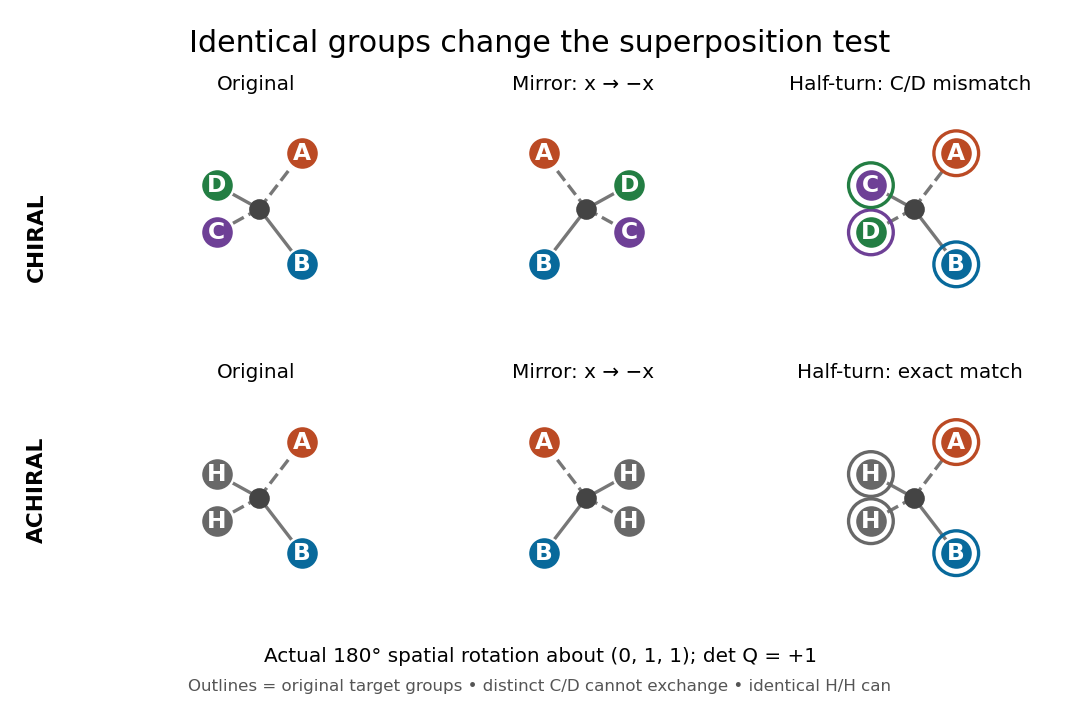
The same spatial half-turn succeeds only when the exchanged groups are identical
. Original model, mirror model and rotated mirror model. Top: the distinct C and D remain mismatched, so the A/B/C/D model is chiral. Bottom: the identical H groups may exchange, so the A/B/H/H model is achiral. The operation is an actual three-dimensional rotation about , with determinant . Details.
For a flexible molecule, also distinguish conformational isomerism from a persistent enantiomer pair. A particular frozen shape may be chiral while ordinary internal motions interconvert mirror shapes. Turning the entire model is always allowed in a spatial comparison; an internal motion must be considered with its actual accessibility and timescale.