Mitosis allocates copied chromosomes to daughter cell nuclei. The spindle apparatus aligns sister chromatids before separation in anaphase.
The copying has already occurred during S phase, before mitosis. Nuclear chromosome segregation and cytokinesis, the partition of the cytoplasm, are distinct processes: two daughter cell nuclei can form inside one undivided biological cell.[ref]
The Cell Cycle. Biology 2e by Mary Ann Clark and others; §10.2, Interphase and The Mitotic Phase; Figure 10.5: replication precedes nuclear division, which can occur without cytokinesis
The original cartoon follows a hypothetical diploid animal biological cell with . Its two homologous chromosome pairs are and ; upper- and lower-case letters identify homologues, not dominant and recessive alleles. In prophase and metaphase, each replicated chromosome contains two sister chromatids: four replicated chromosomes contain eight chromatids, rather than eight replicated chromosomes. The X shape depicts two associated copies, not the shape of every chromosome throughout the cell cycle.
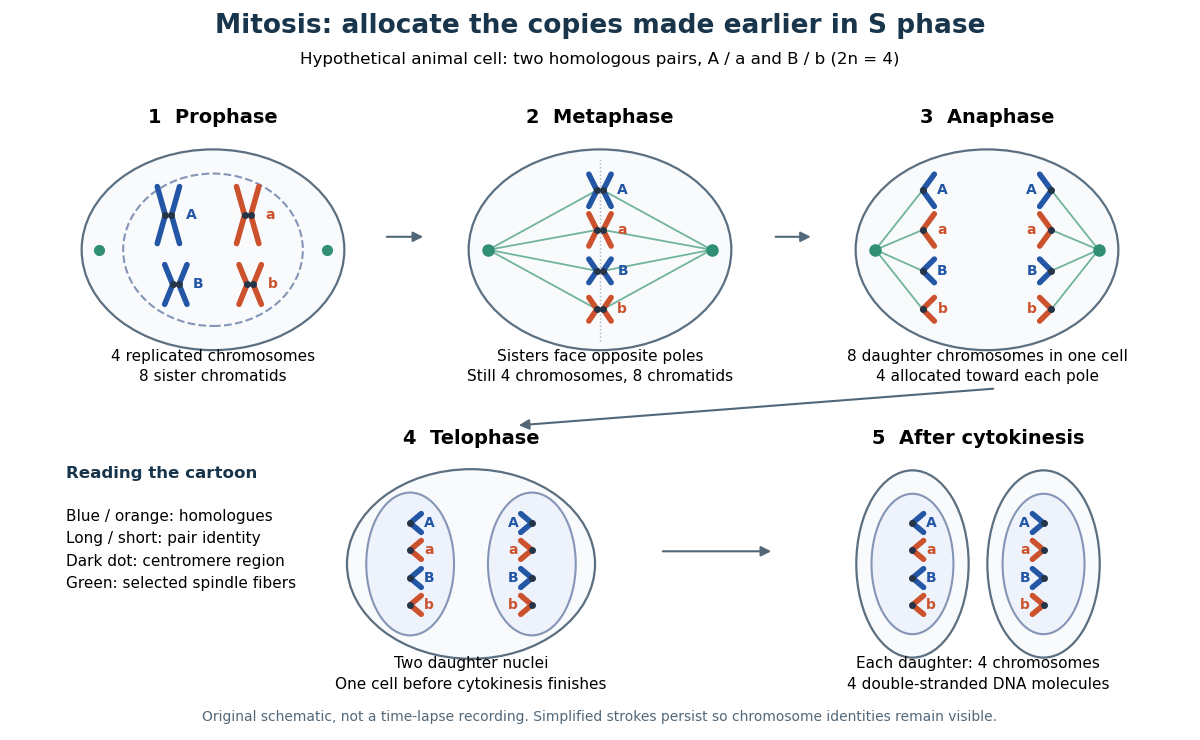
This open mitosis cartoon shows nuclear envelope breakdown and reassembly. Closed mitosis in some yeasts retains the nuclear envelope while daughter chromosomes separate inside it; the cartoon is therefore not a universal cellular architecture.[ref]
The Cell: A Molecular Approach, 2nd edition by Geoffrey M. Cooper. Chapter 8, The Nucleus during Mitosis, Dissolution of the Nuclear Envelope; Figures 8.29–8.30: open and closed mitosis
In open mitosis, nuclear envelope breakdown permits spindle apparatus microtubules to reach kinetochores at centromere regions.
In metaphase, replicated chromosomes align near the spindle apparatus equator, with their two sister chromatids connected through kinetochores toward opposite poles.
In mitotic anaphase, sister chromatids separate into daughter chromosomes moving toward opposite poles.
Release of cohesin-mediated association permits the sister centromere regions to separate. Each former chromatid is then counted as an independent daughter chromosome. This changes the counting convention without making additional DNA copies. For the example, the whole undivided biological cell transiently contains eight daughter chromosomes, four moving toward each pole. Movement toward poles and separation of the poles both contribute to partition in the illustrated animal setting.[ref]
The Cell Cycle. Biology 2e by Mary Ann Clark and others; §10.2, Karyokinesis, Figure 10.6 and Anaphase: release of cohesion, daughter chromosomes and spindle elongation
In open mitosis, telophase includes reassembly of nuclear envelopes around the separated chromosome groups and relaxation of their condensation.[ref]
Count the same hypothetical diploid animal biological cell in three ways: chromosomes, double-stranded DNA molecules, and nuclear DNA amount. Assume one continuous double-stranded DNA molecule per unreplicated chromosome or replicated chromatid, complete S phase, and no losses or mutations. Exclude mitochondrion DNA. Here is the size of one haploid set, and is its unreplicated nuclear DNA amount, as defined in cell-cycle DNA content. A double-stranded DNA molecule counts as one, despite containing two strands.
| Stage and compartment | Chromosomes | Double-stranded DNA molecules | Nuclear DNA amount |
|---|---|---|---|
| One G1 phase parent | 4 unreplicated | 4 | |
| One prophase or metaphase biological cell | 4 replicated | 8 in 4 pairs of sister chromatids | |
| Whole undivided anaphase biological cell | 8 separated daughter chromosomes | 8 | total |
| One anaphase pole's allocation | 4 daughter chromosomes | 4 | allocated |
| Each daughter after mitosis and cytokinesis | 4 unreplicated | 4 | each |
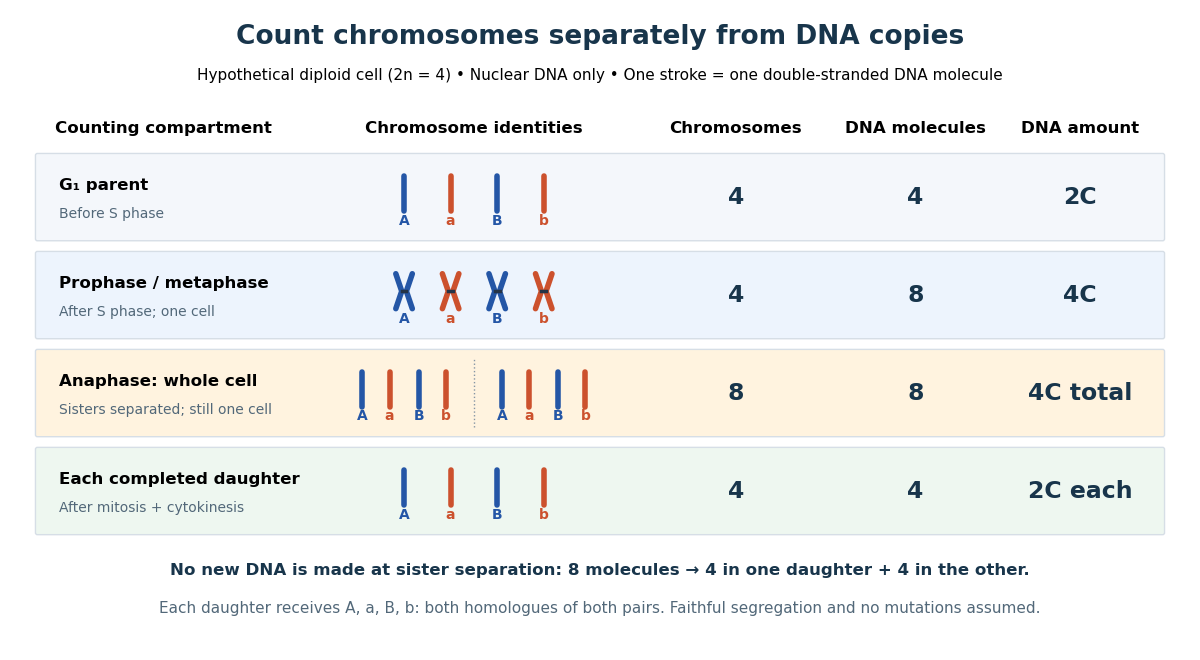
The allocation can be checked copy by copy. DNA replication turns into , into , and similarly for . One daughter receives and the other . Each therefore inherits the same four chromosome identities and the same gene and allele content as the unreplicated parent, under the stated assumptions. Across both daughters there are DNA molecules and : partition conserves the material present after S phase.
The transient whole-cell count of eight does not mean that each daughter's ploidy has doubled. Each completed daughter is diploid, containing both homologues of each homologous chromosome pair. This differs from separating homologous chromosomes during meiosis I. Faithful mitosis preserves a nuclear genome through growth and renewal; equal inherited genes need not imply equal gene expression or equal cell fate. Mutations or chromosome segregation errors can break the ideal inheritance pattern.
The spindle checkpoint can delay anaphase while kinetochore attachment is incomplete. This couples progression to the state of the spindle apparatus, rather than requiring every biological cell to separate its sister chromatids after a fixed waiting time. Alignment in a picture alone is not a demonstration that this control is satisfied.[ref]
Control of the Cell Cycle. Biology 2e, §10.3, Regulation at Internal Checkpoints, Figure 10.11 and The M Checkpoint
A checkpoint component participating in kinetochore-associated signalling and mitotic checkpoint complexes.
A checkpoint regulator involved in attachment surveillance and inhibitory complexes controlling anaphase-promoting complex–Cdc20.
A checkpoint component participating in inhibition of Cdc20 as part of the mitotic checkpoint complex.
A protein assembly that inhibits productive anaphase-promoting complex–Cdc20 activity while kinetochore-associated checkpoint signalling remains active.
In 1995, Conly L. Rieder, Richard W. Cole, Alexey Khodjakov and Greenfield Sluder tested whether an unattached kinetochore supplies the inhibitory signal delaying anaphase. Living PtK1 biological cells on glass coverslips were mounted in Rose chambers at –. An inverted microscope with a objective recorded differential interference contrast microscopy video. A pulsed laser focused through that objective destroyed selected chromosome regions. The readout was chromosome movement and anaphase onset before and after surgery.[ref]
The checkpoint delaying anaphase in response to chromosome monoorientation is mediated by an inhibitory signal produced by unattached kinetochores by Conly L. Rieder and others. pp. 941–942, Abstract and Materials and Methods: Cell Culture; Laser Microsurgery and Video-enhanced Light Microscopy
Destroying the last unattached kinetochore permitted anaphase without that chromosome aligning. Cutting chromosome arms served as a damage control: progression still awaited attachment of the last naturally one-pole-attached chromosome. Correlative electron microscopy checked the absence of the targeted kinetochore. Together these results located an inhibitory activity in or near the unattached kinetochore, rather than establishing a requirement for alignment itself.[ref]
The checkpoint delaying anaphase in response to chromosome monoorientation is mediated by an inhibitory signal produced by unattached kinetochores by Conly L. Rieder and others. pp. 943–947, arm-cutting control, Table I, Figures 1, 5 and 6; destruction of the last unattached kinetochore and correlative electron microscopy
This intervention localized control; it did not identify every signaling molecule or guarantee faithful inheritance after damage. The cultured PtK1 preparation differs from the hypothetical cartoon. Neither the cartoon nor this experiment establishes identical control in every species.


