Mathematical and computational models connect neural mechanisms, measured responses and proposed information-processing functions. Their predictions require comparison with experiments; matching observations does not uniquely identify the biological mechanism.
Updating an internal position or heading estimate from self-motion signals, such as angular velocity and translation. In an ideal planar case, and . Integrating biased or noisy inputs accumulates errors, motivating correction by landmarks and other external cues.
A dynamical neural-network model whose activity tends toward stable states or sets. Recurrent excitation and inhibition can maintain a representation after the original input ends. The model must specify stability and noise consequences to predict behavior.
A localized population-activity pattern in a network with a continuous family of possible represented positions. Noise can shift the pattern's center, producing drift in a remembered continuous variable while the pattern remains present. This yields testable relationships between delay activity and report errors.
A Gabor filter has a kernel formed by multiplying a Gaussian function by a sinusoid or a complex oscillation. In two-dimensional image processing, its orientation and spatial frequency select local image structure; evaluating the kernel's translated dot product with an image is spatial filtering. The real even example under signed spatial filter model of a simple cell uses a cosine.
There is experimental motivation for this family without making every simple cell an exact Gabor filter. Jones and Palmer fitted two-dimensional Gabor filters to measured spatial and spectral response profiles of simple cells in cat cortex and compared independently estimated parameters as a test of spatial linearity. Their reported residuals supported the approximation in that dataset. The chosen parameters and orientation tuning curve in this article are not extracted from their measurements. [ref]
https://pubmed.ncbi.nlm.nih.gov/3437332/. Jones and Palmer, An evaluation of the two-dimensional Gabor filter model of simple receptive fields in cat striate cortex (1987), primary abstract
A dynamic clamp measures a real neuron's voltage, updates a conductance model in real time and injects the resulting current, for example . It implements a virtual conductance without holding the voltage fixed. It can add artificial synapses, couple real neurons into a hybrid network or test how a voltage-dependent conductance affects excitability. Sampling delay and the injection site limit fidelity to spatially distributed biological channels.
For a directed three-neuron rate ring , the linearization has characteristic equation , where . Positive loop gain has strict linear asymptotic stability for . Negative loop gain has it for ; at a complex pair crosses the imaginary axis at frequency . The saturating cubic gives a supercritical Hopf bifurcation under an ordinary loop-gain variation. This directed system does not inherit the energy-descent property of a symmetric Hopfield network.
The leaky integrate-and-fire model combines a passive equation for membrane potential with a firing rule. Between events, inward-positive applied electric current obeyswhere is membrane capacitance, is the leak conductance, is the corresponding electrical resistance, and is the leak reversal potential. Here the leak conductance is constant. The time constant describes passive relaxation. When first reaches a threshold from below, record an action potential event and reset to . In the version used here, hold for a fixed neuronal refractory period , then resume integration. See 1.3 Integrate-And-Fire Models.
For constant , with at the start of an integration interval and , the exact subthreshold solution isThe equilibrium point of this passive equation is . Subtracting leaves , explaining the exponential function. This solution applies only until a threshold event or a change in . Starting below threshold, constant input produces repeated events if ; if , the threshold is approached asymptotically and never reached at finite time.
For a worked example, chooseThese imply and . All these parameters are illustrative model choices, not measurements from a particular neuron. With , Ohm's law gives and hence . ThusAt threshold, , so the first event occurs after . Each subsequent cycle includes the neuronal refractory period, givingThis is the ideal sustained firing rate; the first-event latency is , not .
With instead, and . From the same initial state, stays below : no events occur, however long this current is held. The critical sustained current is ; equality gives asymptotic approach rather than finite-time firing.
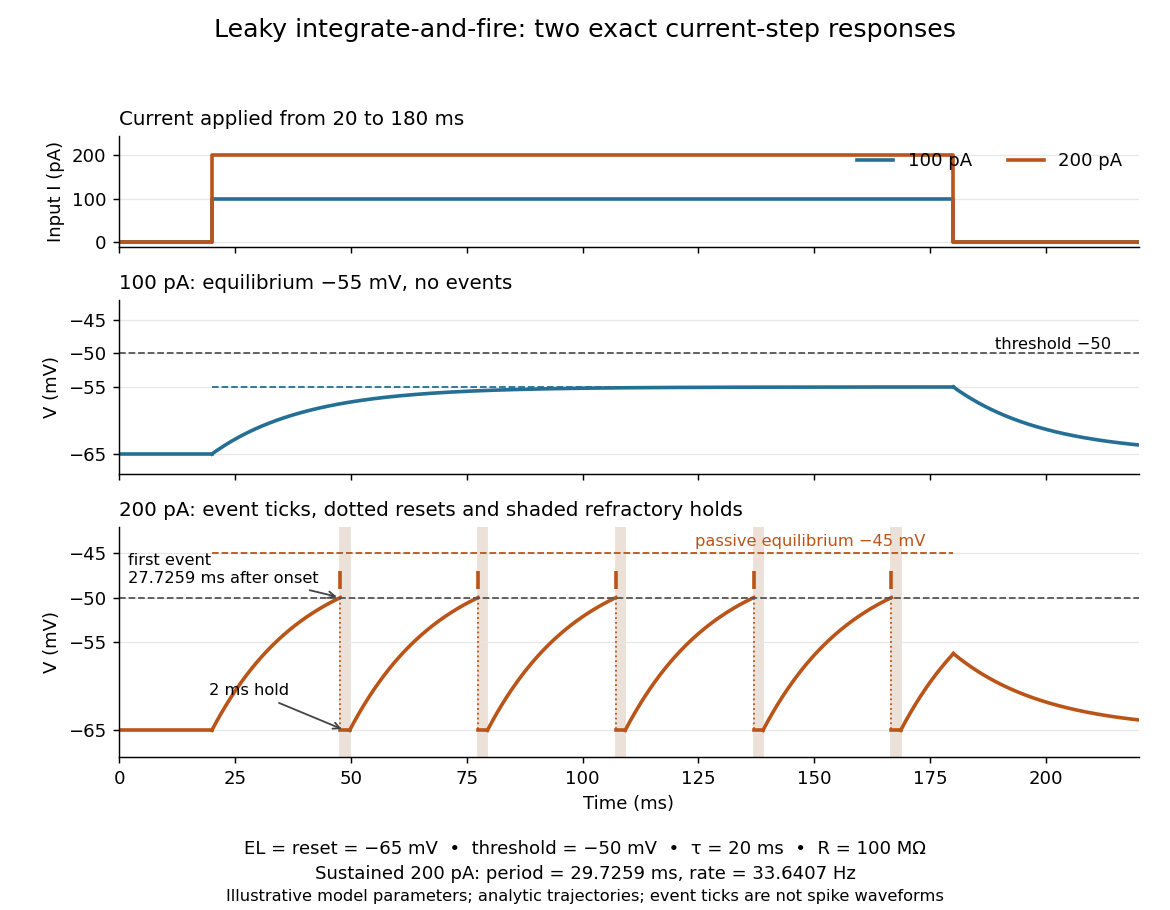
Exact leaky integrate-and-fire responses to two current steps
. Both inputs start at and end at . A step approaches without firing; a step produces threshold events separated by after the first. Orange ticks mark events, and shaded intervals mark the reset hold. The dashed level is the stronger input's passive equilibrium, which the reset trajectory never reaches. These are analytic model trajectories, not recordings or biological spike waveforms. Details.The leak gives old inputs progressively less influence, while capacitance prevents an ordinary finite electric current step from changing instantly. This combination makes the leaky integrate-and-fire model useful for exploring input summation, event timing and network activity at low computational cost. Its fixed parameters and reset omit the evolving voltage-gated ion channels of the Hodgkin-Huxley model, spatial integration in dendrites and mechanisms of neural adaptation. Treating a synapse as a prescribed also omits its voltage-dependent driving force unless a conductance term is added. See 1.4 Limitations of the Leaky Integrate-and-Fire Model and constant-input firing rate of a leaky integrate-and-fire neuron.
For , reset and no explicit refractory interval, define and . Constant current givesThe threshold is approached only asymptotically at . At large current, . Adding an absolute neuronal refractory period changes the denominator to and makes the firing rate saturate rather than grow without bound.
A conductance-based Hodgkin-Huxley model couples membrane potential to voltage-dependent channel-gating variables. It explains generation of action potentials through regenerative and opposing ionic electric currents, while its parameters and channel assumptions determine its biological domain of validity.
In the classical model, describes sodium activation, describes availability against sodium inactivation, and describes potassium activation. Each follows two-state ion-channel gating, with its own voltage-dependent rates. The available electrical conductances areThe barred quantities are maximum electrical conductances. The factors have the interpretation of independent permissive gates in an ion channel: three activation factors and a distinct inactivation-availability factor for sodium, and four identical activation factors for potassium. Large means availability; small means inactivation. These are model assumptions, not a literal structural description of every ion channel. See Gerstner, Kistler, Naud and Paninski, Neuronal Dynamics (2014), §2.2: model definition and stochastic opening.
With inward-positive electric current, a single-compartment form isHere is membrane capacitance, is imposed inward electric current, is leak electrical conductance, and each is a reversal potential. Use consistent units, and either whole-compartment quantities throughout or quantities per membrane area throughout. Opening changes electrical conductance; the reversal potential and present membrane potential determine the associated electric current. Coupling this equation to the voltage-dependent gates makes a generally nonlinear system of ordinary differential equations; a gate's fixed-voltage limit alone does not specify its evolving state during an action potential.
The original quantitative account is [ref]
https://pmc.ncbi.nlm.nih.gov/articles/PMC1392413/. Hodgkin and Huxley (1952), A quantitative description of membrane current and its application to conduction and excitation in nerve, Journal of Physiology 117, 500–544, doi:10.1113/jphysiol.1952.sp004764
. The contrast with the leaky integrate-and-fire model is useful: here an action potential emerges from evolving ionic electric currents, whereas the simpler model records a threshold event and imposes a reset.Replacing the fast activation gate by , taking and assuming constant reduces the Hodgkin-Huxley model to equations for when . Indeed satisfies , so and . The FitzHugh-Nagumo model additionally simplifies the two resulting response functions to a cubic activation equation and a linear recovery equation.
For , with rapidly increasing saturating activation , the zero-current nullcline satisfies in the physical strip. The left side increases strictly, so it defines one height for each voltage. Since , its slope is . Rapid activation can make negative between two positive-slope current regimes, giving two descending attracting branches and an ascending repelling branch in the voltage–recovery phase plane. Sufficient activation steepness is a parameter condition; the shape is not forced by monotonicity alone.
The symmetric two-neuron rate model has nonnegative activity and saturating recurrent input. Every equilibrium has : otherwise monotonicity of gives a contradiction. With positive parameters it has three distinct equilibria exactly when , namely zero and . The lower positive equilibrium is a saddle and the origin and upper equilibrium are stable nodes. The resulting two attracting activity levels model a persistent switch rather than a spiking waveform.
A stimulus passes through a linear temporal or spatial filter, then a nonnegative nonlinear rate function. A conditionally Inhomogeneous Poisson process generates spikes at that rate. The filter and nonlinearity can be fitted from data and tested on held-out trials. Refractoriness and spike-history correlations require extensions beyond this basic cascade.
For a stimulus-conditioned Inhomogeneous Poisson process, the event log-likelihood is the displayed expression. A causal filter expansion can be fitted by maximum likelihood estimation, with a smoothness or size penalty and held-out validation. The integral term penalizes predicted spikes that did not occur; fitting only stimulus values at observed spikes omits this essential part.
Average the stimulus history preceding each observed spike, after removing the stimulus mean. With white Gaussian stimulation and a suitable one-filter encoding model, the result is proportional to the relevant linear filter. An even nonlinearity can make the average vanish despite strong stimulus dependence, so averaging alone is not universally sufficient.
How neural responses represent variables relevant to an organism. A coding claim specifies both which response features carry information and how a downstream system can use them.
Dependence of a neural response on combinations of task variables. A cell can carry information about an object in a context and at a sequence position rather than encode only one of these variables.
The number of recorded action potentials in a specified interval. A count is a nonnegative integer; a fitted firing rate or an expected count need not be an integer.
The number of action potentials per unit time, interpreted as an average over a stated window or as an intensity estimated from a spike train. Window size changes which temporal information remains visible.
A group of neurons whose coordinated activity and learned interactions can represent or participate in an experience. An assembly can overlap with assemblies for other events; it need not assign one private neuron to each memory.
Suppose storing activities changes a matrix by . Any permutation of the activities leaves this sum unchanged. Therefore the update alone cannot distinguish an episode from its reversal. This is a restriction on the stated order-insensitive update, not on all Hebbian learning: trace learning, an evolving context or directed transitions can introduce order information.
An account of regional specialization in terms of the complexity and conjunctions represented, rather than a strict division between perception and memory. The feature-conjunction account of perirhinal cortex proposes object-level combinations that resolve shared-feature ambiguity; higher-order relations can require further interactions.[ref]
Perirhinal cortex resolves feature ambiguity in complex visual discriminations by Timothy J. Bussey and others. 2002, model predictions and controlled feature-ambiguity contrast
A neuron active preferentially at a particular part of a temporally extended task or interval. Temporal selectivity can coexist with selectivity for location, behavior and sequence identity; it is not a claim that the cell is an isolated clock.
A representation of relations among locations or task states that can support inference beyond memorized stimulus–response pairs. The represented space need not be physically spatial. A cognitive-map hypothesis specifies which states and relations are encoded and what behaviour can use them.
A hippocampal population event involving a sharp wave and fast ripple oscillation, often associated with internally generated ensemble activity. Selective interruption can test its contribution to memory, but disrupting an event does not by itself identify the content or computational role of each participating sequence.[ref]
Selective suppression of hippocampal ripples impairs spatial memory by Gabrielle Girardeau and others. Abstract; Nature Neuroscience 12, pp. 1222–1223, post-training ripple suppression
A representation of position or orientation in an external reference frame. Transforming a retinal direction to a world location generally needs eye position, head orientation, self-location and depth or scene geometry. A label in world coordinates is a description of the code, not an explanation of how it develops.
A neuron selective for a viewed location in external space. In the primate recordings motivating the term, eye-position and locomotion measurements distinguished the looked-at part of the environment from the animal’s self-location and head direction.[ref]
Spatial view cells in the primate hippocampus by Edmund T. Rolls and others. Abstract; pp. 1789–1794, active locomotion, eye position and allocentric spatial-view responses
A neuron whose activity is spatially selective for the animal’s own location under specified conditions. Its field can depend on environment, task and sensory context; a visual view and self-location must be disentangled experimentally.
A change in a hippocampal spatial representation across environments or contexts. Models distinguish changes in firing rates, field locations and the relationships among simultaneously recorded units; visual cue changes need not produce one universal kind of response.
A neuron whose firing varies with the orientation of the head relative to the environment. Preferred direction must be distinguished from gaze direction and self-location. Landmark rotation and cue-removal experiments test the visual anchor of this code.[ref]
Rhythmic variation in neural signals. Frequency-band averages can obscure brief events; the timing and duration of bursts can matter independently of mean spectral power.
A neural rhythm in the frequency range conventionally called theta. In rodent hippocampal experiments it provides a temporal reference for comparing the firing of local and remote cells. A matching rhythm does not alone identify the direction or necessity of communication.
A neural oscillation in the frequency band conventionally termed beta, below gamma. Its functional interpretation depends on task, site and temporal structure rather than on frequency alone.
A neural oscillation in a relatively high-frequency band conventionally termed gamma. Exact band boundaries vary by study and recording method.
An extracellular voltage reflecting weighted contributions from nearby and sometimes more distant neuronal currents. Its spatial sensitivity depends on anatomy, electrode placement and signal properties; it is not simply the firing rate of the nearest cell.
Inferring a stimulus, task state or behavior from neural measurements. Successful decoding demonstrates information accessible to the chosen decoder; it does not by itself establish the neural site's causal necessity, exclusive representation or downstream use.
Representation through the joint activity of multiple neurons. Information can reside in relative activity patterns even when the overall mean activity changes little. Neural decoding tests whether recorded patterns carry accessible information under a specified analysis.
Statistical dependence between neural responses remaining after the modeled task-related mean has been removed. Residual dependence can reflect shared state or omitted task variables as well as biological noise, so its interpretation depends on the conditioning model.
Coordinates describing the joint activity of a neural population, often using one coordinate per cell or fitted latent variable. A trajectory connects states over time. A useful reduced description requires evidence that it retains the neural and behavioral properties relevant to the intended claim.
In the observation model , let be an orthogonal matrix. Replacing by and by leaves unchanged because . Thus reconstruction alone does not give each latent axis a unique biological meaning. A particular stochastic model can restrict this symmetry through its prior and parameter constraints; the algebra does not claim every fitted latent model has every rotational ambiguity.
A proposed lower-dimensional set around which recorded population states are organized. The estimated dimension depends on sampling, noise, preprocessing and the scale of variation. A visually smooth embedding is not by itself proof of an intrinsic biological manifold.
The evolution of a population representation over time. A trajectory estimated after trial averaging or strong smoothing can differ from every individual-trial trajectory; this distinction matters for claims about neural dynamics.
Sustained neural activity outlasting a triggering input. Recurrent network dynamics can support persistent representations, but a sustained average signal can also conceal temporally variable events across trials or cells.
The region and stimulus features whose variation influences a sensory neuron's response. A visual receptive field may include spatially distinct ON and OFF regions; a linear receptive-field kernel is a signed weighting map, while the full response can be nonlinear and depend on stimulus history.
ON and OFF receptive-field subregions distinguish locations by response polarity. In the classic mapping experiment, a bright spot in an ON region increased firing during illumination; illumination in an OFF region suppressed maintained firing and/or evoked a discharge when the light disappeared. If maintained firing was very low, suppression could be hard to see. The recorded decrease alone did not distinguish direct inhibition at a synapse from reduced excitation. [ref]
https://xbio-live.s3.amazonaws.com/narratives/57358/Hubel%20and%20Wiesel%201959_Guided%20paper.pdf. Hubel and Wiesel (1959), pp. 576–577: response polarity and inferential limits
These are functional regions in visual space, not compartments of a cell body.For the toy models here, visual contrast means brightness relative to a positive uniform background : . Positive values mean brighter than background, negative values darker, and zero unchanged. This convention separates spatial structure from the background level. A sinusoid with keeps nonnegative. Different experimental conventions for visual contrast require their own definitions; the toy values below do not specify a historical stimulus intensity.
Representation by spike timing, latency, phase or relative timing across neurons, beyond a chosen count summary. Its interpretation requires a timing reference and a decoder capable of resolving the relevant precision.
A tendency for neural spikes to occur at preferred phases of a periodic stimulus. It supplies timing information without requiring one spike on every cycle. Its precision and usable frequency range depend on the cell population and conditions.
Representation by a neuron's firing frequency or the expected spike count in a chosen time window. The window length and averaging convention matter; equal counts do not imply equal temporal patterns.
A sequence of action potential times, represented mathematically as a point process or a sum of Dirac deltas. Its event counts, intervals and correlations summarize different aspects of neural activity.
An interspike interval is the elapsed time between consecutive action potentials in a spike train. Its probability distribution and dependence on previous activity can reveal a neuronal refractory period even when the average firing rate is unchanged.
For a correctly specified conditional rate, transformed interspike intervals have independent unit-exponential distributions, apart from observation-boundary censoring. Their transforms should be uniform. Distributional checks and serial-correlation checks assess a fitted spike model on held-out data. A history-dependent model must include past spikes in its conditional rate; stimulus-only Poisson spike-train likelihood fitting cannot automatically capture refractoriness.
Articles by others on the same topic


Computational neuroscience is an interdisciplinary field that uses mathematical models, simulations, and theoretical approaches to understand the brain's structure and function. It combines principles from neuroscience, computer science, mathematics, physics, and engineering to analyze neural systems and processes. Key aspects of computational neuroscience include: 1. **Modeling Neural Activity**: Researchers create models to replicate the electrical activity of neurons, including how they generate action potentials, communicate with each other, and process information.