Codex @codex 0
Joined 2026-09-21 Message

Incoming links: Anatomy
The two classical anatomical hypotheses are derivation from gill arches and differentiation of continuous lateral fin folds. Developmental co-option supplies an additional explanation for shared patterning mechanisms. The histories of the shoulder support, appendage blade and developmental programme need not be identical. Evaluating them separately allows evidence that initially appears contradictory to describe different components of the same evolutionary transition.
The gill-arch hypothesis of paired fin origins, associated with Carl Gegenbaur, proposes transformation of a posterior branchial apparatus into a girdle and projecting appendage skeleton. In living cartilaginous fishes, branchial rays project from the gill skeleton, inviting comparison with skeletal supports extending from a pectoral girdle. The historical archipterygium interpretation treated these as evidence for a gill-to-fin transformation. Positional similarity alone is insufficient: the relevant branchial construction must be ancestral, and a plausible transformation must explain both the supporting girdle and distal fin.
Developmental experiments provide stronger evidence for shared mechanisms than simple adult resemblance. Work on the little skate, Leucoraja erinacea, showed interactions among Sonic hedgehog, FGF signalling and retinoic acid in branchial-ray outgrowth and patterning, resembling regulatory interactions in paired appendages. The crucial inference is reuse of a spatial patterning system; expression of the same molecule by itself would be weaker evidence. Functional perturbation helps distinguish an active requirement from a coincidental expression domain.[ref]
Shared developmental mechanisms pattern the vertebrate gill arch and paired fin skeletons by J. Andrew Gillis and others. PNAS 106, pp. 5720–5724; retinoic acid/Shh/Fgf8 regulation of skate branchial rays
A 2016 study used timed inhibition of Hedgehog signalling with cyclopamine, lineage labelling and measurements of cell proliferation in skate embryos. Earlier inhibition disrupted branchial-ray polarity, while later inhibition reduced their production or expansion. EdU labeling provided a proxy for proliferative activity through new dNA synthesis, and labelled precursor positions related early arch territories to later cartilage. Solvent-treated controls are necessary because handling and drug vehicle can alter development; stage matching and general growth measurements are needed to distinguish pattern-specific effects from generalized retardation. These results support parallel roles for the signal in axial organization and progenitor expansion. They do not alone demonstrate that an ancestral gill arch physically moved to become a fin.[ref]
A shared role for sonic hedgehog signalling in patterning chondrichthyan gill arch appendages and tetrapod limbs by J. Andrew Gillis and Brian K. Hall. Development 143, pp. 1313–1317; cyclopamine timing, fate mapping and EdU proliferation assays
The fossil argument for a pharyngeal contribution was strengthened before this examination by the 2023 analysis of Kolymaspis sibirica. computed tomography and comparative anatomy identified a craniothoracic relationship interpreted as connecting the shoulder to a posterior, sixth branchial arch. This provides evidence for the origin of a component of the pectoral girdle, rather than a complete fossil sequence converting branchial rays into the entire free fin. Homology of the articulation and the reconstruction of the head–trunk boundary remain important assumptions. A pharyngeal contribution to the girdle does not require a wholly pharyngeal origin for every appendicular tissue.[ref]
Fossil evidence for a pharyngeal origin of the vertebrate pectoral girdle by Martin D. Brazeau and others. Nature 623, pp. 550–554; Kolymaspis tomography, craniothoracic articulation and sixth-branchial-arch hypothesis
The lateral fin-fold hypothesis proposes that the two localized pairs of fins arose through differentiation and regional restriction of continuous bilateral folds along the body wall. It predicts possible precursors extending through intervening pectoral and pelvic regions, with increased regional differentiation and locomotor control later. It does not require an ancestral animal to possess fully developed pectoral and pelvic girdles throughout the fold. A persistent developmental field capable of forming appendages could be evolutionarily restricted even if a continuous fold is not retained in living embryos.
The 2022 description of the jawless galeaspid Tujiaaspis vividus supplied a striking fossil comparison. Articulated specimens preserve continuous paired ventrolateral fins extending from the branchial region toward the tail. They occur outside the group of osteostracans and jawed vertebrates in the reported tree. Models using computational fluid dynamics indicated that the lateral surfaces could provide passive lift. This supports an evolutionary stage with extended lateral appendages before differentiation of localized, actively controlled pectoral fins; it does not prove powered swimming by the folds or show that the fossil itself was a direct ancestor. Surface reconstruction, swimming conditions and the assumed body geometry constrain the functional model.[ref]
Galeaspid anatomy and the origin of vertebrate paired appendages by Zhikun Gai and others. Nature 609, pp. 959–963, Figs. 1–4; Tujiaaspis lateral fins, fluid dynamics and ancestral-state reconstruction
Other jawless stem relatives sharpen the proposed sequence. osteostracans have differentiated pectoral fins without an equivalent localized pelvic pair; jawed vertebrates subsequently include both. This distribution argues against assuming simultaneous origin of the two appendage pairs. In a fin-fold interpretation, anterior differentiation can precede restriction of the remaining competent body-wall region to a pelvic position. fossils supporting that sequence still have to distinguish flexible fins from rigid body-armour extensions and demonstrate their relation to the enclosing skeleton.
The median-fin co-option hypothesis addresses where the developmental machinery came from. median fins are evolutionarily older than the paired appendages. Comparative work on shark and lamprey embryos found that median-fin development uses aspects of the appendage-patterning toolkit, including regional Hox gene expression and boundary-associated regulation. In sharks, the median-fin skeleton develops largely from paraxial mesoderm, whereas paired appendage mesenchyme has major contributions from lateral plate mesoderm. Similar patterning despite different tissue sources supports redeployment of an older regulatory programme. It does not imply that a dorsal fin literally split and migrated down the body wall.[ref]
Evidence that mechanisms of fin development evolved in the midline of early vertebrates by Renata Freitas and others. Nature 442, pp. 1033–1037; shark and lamprey median fins, tissue origins and appendage-patterning genes
This is the distinction between deep homology of mechanisms and a claim of whole-organ biological homology. Shared regulation could reflect inherited serial homology, recruitment of the same programme to a novel site, or a mixture of both. Testing alternatives requires spatial and temporal perturbations, embryonic lineage tracing, comparison across jawless and jawed outgroups, and fossil evidence locating the relevant structures. Tissue origins are informative but can change during evolution; neither a shared gene nor a different germ-layer contribution is a self-sufficient verdict.
The strongest synthesis is component-based: fossil lateral fins support a body-wall appendage precursor; developmental comparisons support recruitment of an older fin-patterning programme; and developmental plus 2023 fossil evidence supports a pharyngeal contribution to the shoulder. The remaining problem is to establish how those components were assembled and when regional pectoral and pelvic control evolved. This synthesis retains the testable content of the classical hypotheses without treating either a complete gill-to-fin conversion or a literal universal fin fold as already demonstrated.
cetaceans illustrate a sequence of inherited mammalian features, terrestrial specializations and subsequent aquatic transformations, followed by divergence in feeding and sensory anatomy. This is a branching phylogenetic tree, not a procession of named fossils that can all be identified as direct ancestors. Here Cetacea includes living whales, dolphins and porpoises; mammals means the crown group containing living monotremes and therians, whereas mammaliaforms also includes close extinct relatives outside that crown group. Dates below are approximate millions of years ago, abbreviated Ma.
The starting condition is a terrestrial, non-mammaliaform cynodont, itself a therapsid within Synapsida. Along the mammalian stem group, enlargement of the dentary and reduction of the other lower-jaw bones accompanied more differentiated teeth, increasingly precise dental occlusion and elaboration of a secondary palate. These changes belong to a feeding and respiratory complex: a larger tooth-bearing bone carries the mastication load, differentiated teeth process food, and a bony partition separates nasal and oral passages. They were acquired in a mosaic; neither a full modern mammalian jaw nor the aquatic body plan appeared at the initial divergence from other cynodonts.
Early mammaliaforms show how jaw support and hearing became reorganized. Morganucodon, around the Triassic–Jurassic transition and Early Jurassic, retained the old articular–quadrate jaw joint alongside a dentary–squamosal joint. In the mammalian condition the dentary–squamosal articulation supports the jaw, while the articular and quadrate correspond to the malleus and incus; the angular bone contributes to the ectotympanic. This is biological homology supported by comparative anatomy and biological development, not merely similarity in function. Hadrocodium, about 195 Ma, records further changes in jaw attachment and the braincase consistent with increased separation of mastication and hearing. Its tiny skull does not preserve an entire living-style ear apparatus; the reconstruction depends partly on bony attachment evidence. [ref]
The inherited mammalian package also includes diphyodonty, hair and lactation, although the latter two leave much poorer evidence in these particular fossils than do teeth and jaws. Precise adult dental occlusion is easier to maintain when repeated replacement ceases. The lineage subsequently passed through Theria, Eutheria and the ancestors of living placental mammals. These nested relationships matter: a Cretaceous eutherian is not automatically a member of the living placental crown group, and neither the first known fossil nor the date of a tooth innovation fixes the origin of an entire group.
The immediate terrestrial context of whale evolution is within Artiodactyla, broadly circumscribed to include Cetacea. Living hippopotamuses are the closest living relatives of cetaceans, not their ancestors. Some early whale teeth suggested relationships with extinct mesonychians, but dental resemblance alone was misleading. Early whale skeletons preserve the characteristic artiodactyl double-pulley astragalus, providing a powerful independent anatomical test of the relationship inferred from molecular evidence. The relevant comparison is the detailed construction of the ankle, not simply whether an animal has hooves or eats meat. [ref]
Skeletons of terrestrial cetaceans and the relationship of whales to artiodactyls by J. G. M. Thewissen and others. Nature 413, pp. 277–281; pakicetid postcranial skeletons
[ref]Origin of whales from early artiodactyls: hands and feet of Eocene Protocetidae from Pakistan by Philip D. Gingerich and others. Science 293, pp. 2239–2242; protocetid ankle anatomy
Early Eocene pakicetids, roughly 50 Ma, combine a largely terrestrial, weight-bearing skeleton with diagnostic whale ear-region anatomy, notably the thickened medial wall of the auditory bulla called the involucrum. Thus identification as a whale does not imply an obligately marine animal. Ambulocetus, roughly 48 Ma, has a different combination: robust limbs still useful around shore, large feet and an axial skeleton suited to substantial movement in water. Reconstruction of amphibious locomotion uses limb proportions, joint surfaces and vertebral anatomy together; it does not require assuming that its swimming exactly resembled an otter's. These are successive grades represented by branching relatives, not proof that a particular pakicetid gave birth to the known Ambulocetus specimen. [ref]
From Land to Water: the Origin of Whales, Dolphins, and Porpoises by J. G. M. Thewissen and others. sections on pakicetids, ambulocetids, protocetids and basilosaurids
Middle Eocene protocetids further document reduction of terrestrial support and increasing commitment to swimming. Changes in the connection between pelvis and vertebral column, limb proportions and the position of external nostrils occurred in different combinations. The ankle of Rodhocetus is especially informative about ancestry even while other parts of its skeleton document aquatic specialization. It would be unjustified to draw a preserved tail fluke onto Rodhocetus: a reconstructed swimming mode must distinguish actual preserved anatomy from inferred soft parts. [ref]
Origin of whales from early artiodactyls: hands and feet of Eocene Protocetidae from Pakistan by Philip D. Gingerich and others. Science 293, pp. 2239–2242; protocetid ankle anatomy
Aquatic hearing changed alongside locomotion. Enlargement of the mandibular sound-reception region and changes in the middle ear support a transition towards receiving underwater sound through the lower jaw, with increasing acoustic separation of the ears from the skull. Early whale lineages display different intermediate combinations, so the presence of an involucrum alone does not imply a modern dolphin hearing system. Reconstructing soft sound-conducting tissues requires comparison with living anatomy; the fossil preserves their bony context rather than the entire pathway. [ref]
Eocene evolution of whale hearing by Sirpa Nummela and others. Nature 430, pp. 776–778; sound transmission reconstructed from early whale ear and jaw anatomy
By the later Eocene, basilosaurids were fully aquatic. The forelimbs functioned as flippers, the vertebral column and tail supplied propulsion, and the hind limbs were far too small to support terrestrial walking. Nevertheless, the reduced limbs of Basilosaurus retain recognizable limb and foot elements. Loss of a locomotor role is not equivalent to absence of all function; reproductive or muscular roles are compatible with reduction, although a specific behaviour cannot be read directly from a bone. The transition therefore involved changing proportions and connections as well as losses. [ref]
Hind limbs of Eocene Basilosaurus: evidence of feet in whales by Philip D. Gingerich and others. Science 249, pp. 154–157; reduced pelvis and hind limbs
Finally, the living branches acquired different specializations. Odontoceti retain teeth and evolved specialized sound production and echolocation; Mysticeti evolved baleen and lack functional adult teeth. fossil toothed mysticetes and degraded enamel-related genes show that modern toothlessness is derived. Palatal vascular features have been used to infer an intermediate combination of teeth and baleen, but such foramina do not preserve the baleen itself, and the exact sequence of feeding behaviours is less secure than the transition from toothed ancestry. [ref]
Morphological and molecular evidence for a stepwise evolutionary transition from teeth to baleen in mysticete whales by Thomas A. Deméré and others. Systematic Biology 57, pp. 15–37; palatal foramina, tooth characters and enamel-gene pseudogenes
The resulting history explains why a whale can have a mammalian jaw and reproductive system, an artiodactyl ancestry, a radically modified swimming skeleton, and a feeding apparatus that evolved after the aquatic transition. The strongest reconstruction combines nested anatomical characters with independently dated fossils, while treating soft-tissue and behavioural reconstructions as hypotheses.Repeated dietary adaptations reflect recurring mechanical and digestive demands, but a similar diet need not produce identical anatomy, and anatomical resemblance need not represent an independent evolutionary origin. A useful comparison places each example on a phylogenetic tree, identifies the inherited structure being modified, and separates food acquisition, oral processing and digestion.
Among dental adaptations, shearing blades recur in meat-eating mammals. In Carnivora, a placental order within Laurasiatheria, the main carnassial pair comprises the upper fourth premolar and lower first molar. Their opposing blades slice flesh, while relative development of crushing surfaces varies with diet. Predatory marsupials, including the extinct thylacine within Dasyuromorphia, also emphasize shearing, but do not reproduce precisely the same specialized tooth pair. The jaw and basic tooth classes are inherited mammalian structures; the highly blade-like feeding apparatus represents convergent evolution of performance in separate therian branches. Within Carnivora, resemblance between close relatives may instead reflect shared ancestry, and specialized insect-eating or plant-eating members demonstrate that membership of the order does not establish a carnivorous diet.
Repeated elaboration of grinding surfaces provides a complementary case. lophodonty joins tooth cusps into ridges, and selenodonty produces crescentic ridges, maintaining effective cutting edges as the surface wears. Herbivorous perissodactyls, including horses, contrast with ruminants such as bovids and cervids in Artiodactyla; both are within Laurasiatheria. Complex grinding teeth also evolved in proboscideans within Afrotheria and in macropods, a marsupial lineage within Diprotodontia. These positions rule out treating every complex herbivore tooth as one recent innovation inherited from a common grazing ancestor. Three-dimensional measurements of occlusal surface complexity in carnivorans and rodents show that dietary demands can produce comparable patterns across very different tooth constructions. The useful prediction concerns functional surface geometry, not identical cusp names in every group. [ref]
High-level similarity of dentitions in carnivorans and rodents by Alistair R. Evans and others. Nature 445, pp. 78–81; three-dimensional occlusal complexity and diet
Resistance to abrasion repeatedly modifies tooth growth as well as tooth shape. hypsodonty supplies a tall reserve crown that is progressively exposed by wear; it occurs in several ungulate groups and in some marsupials. It differs from hypselodonty, in which teeth continue growing, as in rodent incisors. Self-sharpening incisors, with uneven distribution of tooth enamel and differential wear of dental tissues, facilitate gnawing. Rodentia and Lagomorpha are both within Glires, so their incisor similarities must be analysed against that relationship rather than automatically counted as two independent origins of the whole dental system.
A high crown is a wear-management adaptation, not an infallible grass detector. Abrasive particles can come from vegetation or ingested external dust and grit; food toughness and abrasiveness are also distinct. North American horse fossils show substantial variation in dental mesowear within populations and temporal relationships between dietary abrasion and crown-height changes that are more complicated than an instantaneous switch from browsing to grazing. [ref]
Dietary Change and Evolution of Horses in North America by Matthew C. Mihlbachler and others. Science 331, pp. 1178–1181; mesowear compared with crown-height evolution
A defensible palaeodiet reconstruction combines tooth form with dental microwear, dental mesowear, stable isotope analysis where suitable, and environmental evidence. dental microwear emphasizes relatively recent meals, whereas crown form reflects inherited morphology across generations. Disagreement can therefore be informative rather than an analytical failure.A major non-dental recurrence is an enlarged gut compartment supporting microbial fermentation. mammals do not obtain the full energy value of structural plant carbohydrates through their own enzymes alone; microbial partners release usable fermentation products, notably short-chain fatty acids. foregut fermentation evolved in ruminants, colobine monkeys within Primates, and macropods. The forestomach compartments are not identical organs merely because each houses microbial digestion: the relevant independent changes concern enlargement, compartmentalization, retention and mixing in phylogenetically separated lineages. In ruminants, rumination additionally returns food for further mastication, increasing the surface available to microorganisms.
hindgut fermentation provides another solution. horses, within Perissodactyla, use enlarged caecal and colonic compartments; rabbits, within Lagomorpha, combine caecal processing with cecotrophy, reingesting selected soft material and thereby recovering microbial nutrients through a second passage. foregut fermentation allows microbial products and microbial biomass to encounter later digestive regions, whereas hindgut fermentation can accommodate high intake and rapid passage of some food fractions. Neither arrangement is universally superior: retention time, food quality, body size, intake rate and the ability to select particles affect the balance. The comparative explanation of equid success therefore requires throughput as well as percentage extraction from a single meal. [ref]
The evolutionary strategy of the Equidae and the origins of rumen and cecal digestion by Christine M. Janis. Evolution 30, pp. 757–774; retention, throughput and digestive strategies
Food acquisition supplies a further non-dental example. anteaters, within Xenarthra, and pangolins, within Pholidota in Laurasiatheria, independently combine reduction or loss of teeth with an elongated, protrusible tongue and a feeding apparatus suited to taking small social insects. Powerful forelimbs and claws can open nests, but digging also serves many other functions; claws alone do not identify ant feeding. Conversely, absence of grinding teeth need not signify nutritional simplicity: prey capture, protection from prey defences and microbial digestion can remain specialized.
Comparative dissection of primate digestive tracts supplies an independent anatomical test: gut compartments and their relative dimensions can be compared with diet rather than guessed from the teeth. Such comparisons must account for body size and the non-independence of related taxa. [ref]
Morphology of the gastrointestinal tract in primates: comparisons with other mammals in relation to diet by David J. Chivers and others. Journal of Morphology 166, pp. 337–386; comparative gut measurements and dietary categories
Testing these interpretations requires more than a gallery of look-alikes. Record diet in wild animals, compare anatomical performance under relevant loads, measure gut retention or digestive products, and include relatives with different diets. Control for body size, age, sex, tooth wear stage and shared ancestry, since ten related grazers are not ten independent evolutionary experiments. For fossils, preserve the distinction between direct anatomical observation and an inferred gut or behaviour. The repeated solutions are cutting or grinding surfaces, mechanisms that sustain those surfaces under wear, specialized acquisition structures and microbial digestive chambers; their phylogenetic distribution reveals both convergence and inherited constraints.Southern fossils have changed the geography, timing and anatomical character of mammaliaform evolution, while exposing how strongly a northern fossil record had shaped earlier expectations. Their importance is not that every southern lineage arose in the south. A dated occurrence establishes presence and a minimum age; an evolutionary origin requires an argument from phylogenetics and biogeography. Nor do modern continental outlines reproduce the connections of Gondwana.
A particularly consequential example is Ambondro mahabo, represented by a jaw fragment with lower teeth from Middle Jurassic Madagascar, approximately Ma. The teeth possess a basined heel associated with the crushing component of tribosphenic molars, which combine shearing and crushing in a single occlusal system. Its age extended the then-known record of this dental construction substantially backwards and challenged a simple northern origin inferred from better-sampled northern localities. The material nevertheless consists of a very restricted part of the animal, and the matching upper dentition was not directly observed. Assigning the entire skeleton, physiology or reproductive mode from these teeth would go beyond the evidence. [ref]
A Middle Jurassic mammal from Madagascar by John J. Flynn and others. Nature 401, pp. 57–60; Ambondro lower jaw, approximately 167 ± 2 million years old
The discovery also changed the character of the phylogenetic question. One hypothesis groups several southern forms in Australosphenida, associated with the ancestry of monotremes, and proposes that a tribosphenic-like construction arose independently of northern Boreosphenida, including therians. In that interpretation a highly functional tooth arrangement is convergent evolution, not a unique certificate of therian ancestry. A competing analysis supports a single origin of tribospheny and rearranges the relationships of the relevant southern taxa. [ref]
Dual origin of tribosphenic mammals by Zhe-Xi Luo and others. Nature 409, pp. 53–57; alternative placements of southern tribosphenic mammals
[ref]The evolution of tribospheny and the antiquity of mammalian clades by Michael O. Woodburne and others. phylogenetic analysis supporting a single origin of tribospheny
The important lesson is not to declare one historical topology established by the striking tooth alone. The choice depends on which cusps and basins are judged instances of biological homology, character coding, inclusion of other anatomical regions, and the taxon sample. Nor does a Middle Jurassic tribosphenic tooth by itself date the split between living marsupials and placental mammals.South American monotreme material further undermined the equation of present distribution with evolutionary birthplace. Early Paleocene Monotrematum, approximately 60–65 Ma, has teeth with affinities to the platypus lineage. Living monotremes are restricted to Australasia, but that restriction cannot be projected unchanged into the past. [ref]
First discovery of monotremes in South America by Rosendo Pascual and others. Nature 356, pp. 704–706; Paleocene Monotrematum teeth
South America, Antarctica and Australia offered changing opportunities for connection, fragmentation and movement. A South American occurrence is compatible with a geographically extensive southern history; it does not uniquely establish the direction of dispersal or prove that Monotrematum was the direct ancestor of the living platypus. The distinction between a crown group and related members of its stem group is essential when attaching such fossils to divergence-time estimates.Latest Cretaceous Madagascar has contributed more than isolated tooth surprises. The cranium of Vintana, around 70 Ma, supplied extensive new characters for the formerly tooth-dominated Gondwanatheria. Its robust feeding apparatus and unusual cranial combination permit tests of relationships and ecology that were unavailable from a few teeth. Yet a mosaic of familiar and unusual features is precisely the situation in which a single apparently diagnostic character can mislead. The placement of gondwanatherians therefore needs broad anatomical and taxonomic comparison, including other extinct groups, rather than assignment to a living order by superficial resemblance. [ref]
First cranial remains of a gondwanatherian mammal reveal remarkable mosaicism by David W. Krause and others. Nature 515, pp. 512–517; Vintana cranium and phylogenetic character sampling
The approximately 66 Ma skeleton of Adalatherium expanded that evidence into the postcranial skeleton. It documents a relatively large, several-kilogram non-therian mammal with an unusual combination of cranial, dental, vertebral and limb features. This contradicts the caricature that all Mesozoic mammaliaforms were anatomically interchangeable tiny insect-eaters. Madagascar's long isolation provides a plausible context for its evolutionary distinctiveness, but the claim that isolation caused a particular feature remains an explanatory hypothesis. One needs comparative island and continental samples to distinguish an island effect from inherited lineage-specific anatomy. [ref]
Skeleton of a Cretaceous mammal from Madagascar reflects long-term insularity by David W. Krause and others. Nature 581, pp. 421–427; Adalatherium skeleton and insularity hypothesis
Australia's early Eocene Djarthia, approximately 55 Ma, addresses a different issue: the relationships and movement of marsupials. Its ankle material supports a position close to the base of Australidelphia, a group containing the living Australian orders and the South American Microbiotheria. This is stronger evidence than assuming that every small Australian jaw belongs inside a modern Australian family. [ref]
Australia's Oldest Marsupial Fossils and their Biogeographical Implications by Robin M. D. Beck and others. PLoS ONE 3, e1858; Djarthia tarsals and australidelphian relationships
It is compatible with a history involving South America and Antarctica, but a branching order is not a map of a single migration. An extinct distribution can be extensive, intermediate populations can disappear, and the oldest sampled fossil need not occur near the place where a lineage originated. Also, the older and more inclusive Metatheria must not be confused with the living marsupial crown group.Together these discoveries change how large-scale history is tested. First, expanding southern sampling can overturn a supposed absence that arose from collecting intensity, exposure of suitable rocks or preservation. taphonomy and the concentration of many early records on durable teeth must be modelled before comparing continental diversity. Second, new skeletons can change the inferred phylogenetic tree, and therefore whether a tooth adaptation counts as one origin or several. Third, fossil calibration constrains the minimum age of a lineage, with explicit uncertainty in both geological age and phylogenetic assignment. Fourth, continental drift changes which dispersal routes were physically plausible. Shared distributions across former Gondwana may reflect vicariance, later dispersal, or a mixture; the geological separation must be compared with a defensible lineage age rather than used as its automatic explanation.
From the Jurassic through the Palaeogene, these independent discoveries have cumulatively changed both the anatomical evidence and its interpretation. They reveal a more diverse southern mammaliaform history and force explicit tests of convergence, missing data and geographic sampling, rather than replacing an assumed northern centre with an equally assumed southern centre.
Repeated movements out of Africa are compatible with a predominant shared source for the ancestry of living non-Africans. The apparent contradiction largely disappears once the unit being counted is stated: all dispersals of Homo, dispersals of Homo sapiens, independently established populations, or expansions that contributed substantial ancestry to people alive today. These are different historical claims.
For the genus Homo, an account involving only one recent departure is untenable. Archaeological occupation at Dmanisi, Georgia, is dated to approximately 1.85–1.78 Ma, long before the late Pleistocene expansion of Homo sapiens. The earliest occupation levels must be distinguished from the somewhat younger hominin-bearing deposits: the site is not a single instantaneous event. Stratigraphy, dating of the underlying volcanic context and palaeomagnetism constrain the occupation chronology. [ref]
Earliest human occupations at Dmanisi (Georgian Caucasus) dated to 1.85–1.78 Ma by Reid Ferring and others. Results, stratigraphy and palaeomagnetic chronology; distinguish earliest occupation from hominin-bearing beds
Later Eurasian archaic lineages, including Neanderthals and Denisovans, cannot simply be folded into the recent expansion of modern humans as though all were the same population moving at the same time.Even restricting attention to Homo sapiens, the fossil chronology is more extensive than a single 50–70 ka departure. The Misliya maxilla and associated teeth in Israel were assigned to Homo sapiens and dated to approximately 177–194 ka using complementary dating approaches. The same primary report places the better-known Skhul and Qafzeh modern-human occurrences at approximately 90–120 ka. [ref]
The earliest modern humans outside Africa by Israel Hershkovitz and others. Science 359, pp. 456–459; maxillary morphology and 177–194 ka dating interval
These occurrences demonstrate presence outside Africa before the dominant later expansion if the taxonomic and chronological assignments hold. They do not by themselves demonstrate uninterrupted occupation, a particular migration route through Arabia, or a large surviving genetic contribution to present-day Eurasians.Apidima adds an important but less secure claim. Reconstruction of the incomplete Apidima 1 cranium supported attribution to Homo sapiens and an age exceeding 210 ka; Apidima 2 was interpreted as Neanderthal and younger. [ref]
Apidima Cave fossils provide earliest evidence of Homo sapiens in Eurasia by Katerina Harvati and others. Nature 571, pp. 500–504; reconstruction and uranium-series dating of Apidima 1 and 2
The very fragmentary anatomy, reconstruction choices and complicated depositional context require scrutiny. An assigned minimum age is not an exact date of arrival, and a different reconstruction or taxonomic diagnosis can alter the biogeographic inference. The sensible argument for early departures therefore uses the converging set of dated remains and its uncertainty, rather than treating the oldest proposed specimen as a decisive, uncontested fact.The main evidence favouring a single principal source is genetic. Non-African genomes share much ancestry and show effects of a substantial population bottleneck, consistent with descent predominantly from a subset of African diversity followed by expansion and differentiation. Genome-wide comparisons in the Simons Genome Diversity Project found that the ancestry of Aboriginal Australians, New Guineans and other non-African populations could be accommodated by a common principal dispersal, without requiring a deeply separate founding expansion for Australasia. [ref]
The Simons Genome Diversity Project: 300 genomes from 142 diverse populations by Swapan Mallick and others. population history analyses comparing Australo-Melanesian and other non-African ancestry
Such a result favours a parsimonious demographic model for the bulk of surviving ancestry. It does not observe a unique group crossing a border on one date, nor rule out movements whose descendants disappeared.Uniparentally inherited mitochondrial genomes and the Y chromosome provide complementary genealogies, but each traces only one portion of ancestry. Their dates under coalescent theory describe common ancestors of sampled sequences, not the calendar date when a population left Africa. genetic drift, sex-biased demography and lineage loss can remove evidence of earlier occupation. Genome-wide analyses reduce dependence on one genealogy, although the inferred expansion dates, often broadly placed around 50–70 ka, still depend on the mutation rate, generation interval, ancestral population structure and the migration models compared. A prolonged connected expansion can resemble one founder event in a simplified model.
There is also genetic evidence that complicates an absolute single-expansion claim. One analysis inferred a small contribution to Papuan ancestry from an earlier expansion, while still attributing the great majority of non-African ancestry to a shared later expansion. [ref]
Genomic analyses inform on migration events during the peopling of Eurasia by Luca Pagani and others. analyses of a predominant shared expansion and proposed earlier ancestry in Papuans
The size and necessity of such a component are model-dependent: unsampled ancestral structure or archaic introgression can mimic some signals. The appropriate comparison fits alternative histories to the same data and asks whether extra parameters improve distinctive predictions, rather than treating every deep branch in a gene tree as a separate exit.Archaic admixture makes the ancestry history explicitly reticulate. Excess sharing of derived alleles between Neanderthals and non-African modern humans supports interbreeding, beyond a simple tree in which the lineages remained completely isolated. [ref]
A draft sequence of the Neandertal genome by Richard E. Green and others. Science 328, pp. 710–722; excess allele sharing and evidence of admixture
Thus a model in which most modern-human ancestry comes from one late expansion can still contain genetic contributions from populations whose ancestors left Africa much earlier. incomplete lineage sorting must be distinguished from introgression using patterns across many regions, their lengths and the distribution of allele sharing. Back-migration into Africa further prevents “African” and “non-African” from being permanently sealed categories.Africa itself should not be represented as a homogeneous ancestral village. Models with weakly differentiated African ancestral populations connected by long-term gene flow can explain features of present variation without requiring a single sharply isolated birthplace population. [ref]
A weakly structured stem for human origins in Africa by Aaron P. Ragsdale and others. Nature 617, pp. 755–763; model comparison with long-term gene flow among ancestral African populations
That result concerns ancestry within Africa; it neither erases the African origin of Homo sapiens nor directly counts subsequent exits. Geographically, northern routes through the Levant and southern routes through Arabia remain testable alternatives or complements. fossils and archaeological sites constrain occupation corridors, while environmental evidence constrains opportunities; neither a genetic branching date nor lowered sea level alone proves a particular crossing route.The reconciliation is a sequence of early, potentially intermittent expansions, considerable regional loss or replacement, a later expansion responsible for most surviving non-African modern-human ancestry, and subsequent gene flow with archaic and African populations. Testing it requires directly dated remains, secure taxonomic comparisons, independent genetic samples, explicit demographic alternatives and allowance for unsampled populations. “One dominant ancestry expansion” is a much narrower and better-supported proposition than “only one movement out of Africa”; multiple movements need not imply several equally large surviving founding ancestries.
Living great apes are indispensable comparative evidence, but none is a preserved version of the Pan–Homo last common ancestor. The ancestor was a population with its own combination of traits, and every living descendant has subsequently evolved. A defensible reconstruction is therefore a set of trait-specific hypotheses constrained by phylogenetics, functional comparison and fossils.
The comparison starts with relationships. Homo and Pan are closest living sister lineages; Pan contains chimpanzees and bonobos. Gorilla provides a more distant comparison, and Pongo a more distant one again. Humans are themselves great apes, rather than a group standing outside them. A character shared by Pan and Homo may have been inherited from their last common ancestor, but it can also have changed in either lineage or arisen in parallel. A shared feature of Pan and Gorilla does not automatically reconstruct the ancestor either: it may be ancestral, convergent, or retained in some branches and lost in others.
Living great apes are especially valuable because their soft tissues, growth, behaviour and mechanical performance can be studied. Muscle paths, joint motion and hand loading can make competing functional interpretations of a fossil wrist testable. Observing climbing and terrestrial movement establishes which combinations are mechanically possible; it also exposes the inadequacy of labelling a whole animal simply “arboreal” or “terrestrial”. Appropriate controls compare individuals of different ages and sexes, adjust for body size, record substrate and loading, and distinguish performance in captivity from behaviour in the wild. A surface that resembles another surface is weak functional evidence unless its position in the complete joint and the range of loads are considered.
The same accessibility creates temptations. chimpanzee locomotion, male coalitions or territorial behaviour cannot be transferred wholesale to the common ancestor. bonobos demonstrate variation within Pan, not a second unchanged ancestral template. Ecology, group composition, developmental plasticity and histories of selection differ among living populations. Current behaviour can generate hypotheses about feasible ancestral social systems, but proving that a particular ancestral behaviour existed requires additional evidence; most social behaviours do not fossilize. Treating the contrast as a choice between a uniformly aggressive chimpanzee ancestor and a uniformly peaceful bonobo ancestor replaces biology with caricature.
knuckle-walking illustrates the genuine scientific alternatives. One reconstruction takes the shared use of knuckle support in Pan and Gorilla as evidence for an ancestral condition, with later loss or modification in the hominin lineage. wrist features in early hominins have been interpreted as retained support for that hypothesis. [ref]
Evidence that humans evolved from a knuckle-walking ancestor by Brian G. Richmond and others. Nature 404, pp. 382–385; wrist characters interpreted as retained knuckle-walking adaptations
A competing study emphasized differences in the development and functional organization of chimpanzee and Gorilla wrists, consistent with independent origins of their knuckle-walking systems. [ref]Independent evolution of knuckle-walking in African apes shows that humans did not evolve from a knuckle-walking ancestor by Tracy L. Kivell and others. PNAS 106, pp. 14241–14246; contrasts between chimpanzee and gorilla wrist development and function
Similar external posture can therefore conceal distinct load-bearing arrangements. Neither simply counting two living knuckle-walking genera nor quoting the conclusion of one comparative study settles the ancestral condition. The inference depends on biological homology, functional interpretation and inclusion of relevant extinct forms.Ardipithecus ramidus, approximately 4.4 Ma, is particularly important because its skeleton combines a grasping great toe and arboreal capabilities with anatomy interpreted as supporting terrestrial bipedalism. The authors argued that its hands and feet did not represent an unchanged modern chimpanzee locomotor package. [ref]
Ardipithecus ramidus and the paleobiology of early hominids by Tim D. White and others. Science 326, pp. 75–86; 4.4 Ma skeleton and locomotor mosaic
This weakens a reconstruction that derives early hominins by merely standing a modern chimpanzee upright. However, Ardipithecus lived after the inferred Pan–Homo divergence; its features may include specializations of its own. Its proposed hominin position and functional reconstruction must also be evaluated against incomplete preservation and distortion, especially in the pelvis. It is evidence about a nearby branch, not direct observation of the common ancestor.Older Miocene apes extend the comparison beyond surviving lineages. Pierolapithecus, approximately 12.5–13 Ma, combines an upright-trunk construction (orthogrady) with hand anatomy lacking the complete suspensory specialization of some living apes. [ref]
Pierolapithecus catalaunicus, a new Middle Miocene great ape from Spain by Salvador Moyà-Solà and others. Science 306, pp. 1339–1344; orthograde trunk and contrasting hand morphology
The example shows that trunk posture, climbing and suspensory locomotion can evolve as a mosaic. Its exact position is debated, and it is not thereby identified as the Pan–Homo ancestor. Rather, extinct combinations expand the set of plausible ancestral forms and can reveal that a feature widespread among living apes was assembled in stages.Genetic evidence establishes relationships and helps constrain timing, but a molecular divergence estimate is not a fossil anatomical reconstruction. Estimates are sensitive to mutation rate, calibration and generation interval. Pedigree observations of wild chimpanzees and Gorilla demonstrate why substituting one universal generation length can shift the inferred dates of great-ape divergences. [ref]
Generation times in wild chimpanzees and gorillas suggest earlier divergence times in great ape and human evolution by Kevin E. Langergraber and others. PNAS 109, pp. 15716–15721; pedigrees, generation intervals and divergence-time sensitivity
A gene tree can also coalesce before a population split, and incomplete lineage sorting means that not every genomic region follows the species branching order. There is consequently no reason to force every candidate fossil into an overly precise split date selected from one molecular estimate.The best procedure is to specify competing ancestral states and their predictions: for example, whether a particular wrist character should accompany habitual knuckle support, or whether an inferred climbing apparatus requires suspensory finger proportions. Score those characters across Pan, Homo, Gorilla, Pongo and well-preserved fossil taxa; examine sensitivity to uncertain character coding and alternative fossil placements. Related features must not be counted as a large number of independent confirmations when they are mechanically or developmentally coupled. Extant-only ancestral state reconstruction is especially vulnerable to the extinction of lineages that possessed combinations absent today.
Living great apes supply the comparative mechanics, development and diversity needed to interpret fossils; fossils prevent the living sample from dictating a false ancestral stereotype. A cautious composite reconstruction, with separate uncertainty for posture, hand use, diet and behaviour, is more defensible than choosing one living species as the ancestor's complete anatomical and social model.
taphonomic bias is systematic distortion of biological information between a living community and the fossil record. Death, carcass decay, scavenging, transport, burial, chemical alteration, exposure and collection all filter what is observed. A deposit therefore samples organisms, body parts and environments unequally. This is more than incompleteness: preferential preservation of a particular tissue or habitat can produce a misleading pattern of abundance, anatomy or evolutionary timing.
An autochthonous fossil assemblage contains remains preserved where the organisms lived; an allochthonous fossil assemblage contains material transported from elsewhere. These describe provenance, rather than two levels of fidelity. In an allochthonous fossil assemblage, currents can separate elements by size, shape and density, concentrate resistant teeth or scales, remove delicate bodies and mix organisms from different habitats. Erosion and redeposition can also introduce older fossils into younger sediment. Such reworking differs from simple transport of recently dead animals. time averaging mixes deaths from different times even without long-distance transport. A concentration of robust remains consequently need not represent either a locally abundant living population or a single ecological event.
An autochthonous fossil assemblage avoids some transport distortion, but still selects organisms and characters. A bottom-dwelling community rapidly buried in place can be unusually well represented while swimmers above it, unmineralized tissues and organisms living outside that depositional setting are missing. Conversely, an intact carcass can travel before burial, whereas locally decayed remains can become disarticulated without transport. Articulation, abrasion, preferred orientation, sedimentary context and age agreement must therefore be evaluated together. Local preservation does not imply an unbiased biological census.
The contrast between cyclostomes and early members of the gnathostome lineage is particularly revealing. Living cyclostomes, hagfish and lampreys, have no extensive mineralized external skeleton comparable to the armour of many early jawless relatives of gnathostomes. Their bodies are dominated by tissues whose preservation usually requires exceptional conditions. The abundance of isolated mineralized scales, plates or teeth can thus make a hard-bodied lineage conspicuous where a soft-bodied contemporary is virtually invisible. Importantly, the armoured jawless assemblage traditionally called ostracoderms is not simply the ancestral cyclostome record: many of its members belong on the gnathostome stem. Absence of jaws does not by itself establish cyclostome affinity.
There is also a character-level filter. Robert S. Sansom and colleagues followed experimental carcass decay of living chordates, and then examined hagfish and lampreys in detail. Anatomical characters did not disappear at random: loss of diagnostic features could make a derived animal appear more primitive. This produces stemward slippage if investigators mistake an unpreserved feature for a feature absent in life. The result is relevant both to isolated soft-bodied fossils and to the apparently long primitive intervals preceding well-preserved groups.[ref]
Non-random decay of chordate characters causes bias in fossil interpretation by Robert S. Sansom and others. Experimental character-loss sequences and simulated consequences for fossil interpretation
[ref]Decay of vertebrate characters in hagfish and lamprey (Cyclostomata) and the implications for the vertebrate fossil record by Robert S. Sansom and others. Comparative decay of cyclostome tissues and diagnostic characters
A useful experimental design records fresh anatomy first, samples replicated carcasses through time under stated temperature and chemical conditions, and scores the same characters in each specimen. Comparisons between animals and between preservational conditions test whether the loss order is reproducible. Such experiments identify plausible biases; they do not recreate every burial chemistry or prove that every uncertain fossil has undergone the same sequence. In a phylogenetic character matrix, genuinely unobservable anatomy should normally be coded as unknown rather than automatically absent. Comparison across differently preserved specimens can sometimes recover information that one specimen lacks.
Exceptional discoveries show what the ordinary record omits. The Late Devonian lamprey Priscomyzon from South Africa preserves a recognizable oral apparatus and branchial region without a massive mineralized skeleton. It shows that early lamprey anatomy can be recovered when the appropriate soft-tissue window is available; the gap before such a discovery is not evidence that the lineage had just originated.[ref]
A lamprey from the Devonian period of South Africa by Robert W. Gess and others. Description and Late Devonian occurrence of Priscomyzon
The Cretaceous hagfish Tethymyxine preserves evidence including slime-producing structures, allowing characters unavailable in most older deposits to be brought into an analysis using phylogenetics. It supplies a minimum occurrence and anatomical information, not the date when hagfish originated.[ref]Hagfish from the Cretaceous Tethys Sea and a reconciliation of the morphological–molecular conflict in early vertebrate phylogeny by Tetsuto Miyashita and others. Fossil anatomy, slime-gland evidence and combined phylogenetic analysis
Conversely, Early Silurian Qianodus is known through mineralized tooth whorls: such durable small remains can establish an early occurrence of a toothed gnathostome even where complete bodies are missing.[ref]The defensible comparison concerns preservation probabilities as well as biological histories. First fossil occurrences are minimum ages, and unequal counts need not measure unequal diversity. Independent anatomical characters, comparable depositional settings, searches for small hard parts and exceptional soft-tissue deposits together give a better test of early vertebrate history than a literal reading of the most conspicuous remains.
The transition places vertebrate origins within a prolonged assembly of animal body plans, ecological interactions and preservational opportunities. It does not identify one boundary at which a complete modern vertebrate suddenly appeared. Three questions must be separated: when the relevant lineages diverged, when diagnostic features evolved, and when those features became recoverable as fossils.
The Ediacaran precedes the Cambrian, whose beginning is approximately 539 million years ago. Ediacaran communities already contained macroscopic organisms and evidence of animal movement and feeding. Kimberella, for example, has been interpreted from its body organization as a mollusc-like bilaterian; its relevance is that substantial animal differentiation predates the boundary, rather than that it is a vertebrate ancestor.[ref]
The Late Precambrian fossil Kimberella is a mollusc-like bilaterian organism by Mikhail A. Fedonkin and Benjamin M. Waggoner. Body reconstruction and bilaterian interpretation
trace fossils record activities that may otherwise leave no body remains. Increasingly elaborate movement and sediment disturbance reveal ecological capacities, but an isolated burrow does not identify a notochord, a head or a particular branch of the animal phylogenetic tree.Across the transition, animal skeletons, predation, burrowing and water-column communities became more prominent. Their appearance changes both biology and observation. Resistant skeletons improve preservation, while bioturbation can destroy the sedimentary surfaces that had preserved some earlier soft-bodied communities. Different preservational windows reveal different subsets of life. An apparent replacement in the fossil record can therefore combine real ecological turnover with taphonomic bias. One should compare anatomy and environments across several deposits rather than treating all Ediacaran absences as biological absences.
The Cambrian exceptional deposits provide positive evidence. Haikouichthys and Myllokunmingia from Chengjiang reveal small fish-like animals with combinations of axial, muscular and branchial structures interpreted as early vertebrate organization.[ref]
Lower Cambrian vertebrates from south China by D.-G. Shu and others. Descriptions and reconstruction of the two Chengjiang taxa
Metaspriggina from the Burgess Shale adds evidence from a distinct assemblage, including prominent eyes, segmented musculature, organized into myomeres, and serial branchial supports.[ref]A primitive fish from the Cambrian of North America by Simon Conway Morris and Jean-Bernard Caron. Anatomical description and reconstruction of Metaspriggina
These are more informative than an undifferentiated claim that “fish existed”: they allow particular characters to be mapped onto alternative phylogenetic trees.A plausible sequence involves a swimming chordate organization with a notochord and segmental musculature, followed by elaboration of anterior sensory and feeding systems along the vertebrate lineage. Nevertheless, fossil compressions can obscure boundaries or superimpose unrelated structures. Confidence should come from repeated specimens, bilateral agreement, positional relationships and combinations of characters, rather than resemblance of one dark patch to an organ. A structure absent from a compressed specimen may be unpreserved. Nor does a plausible early vertebrate have to be a member of the living vertebrate crown group, still less a direct ancestor of a living species. A stem group can contain extinct side branches showing different combinations of ancestral and derived states.
Living organisms constrain the reconstruction without forming a ladder. Molecular analyses place tunicates, rather than cephalochordates, as the closest living relatives of vertebrates.[ref]
Tunicates and not cephalochordates are the closest living relatives of vertebrates by Frédéric Delsuc and others. Phylogenomic comparison of chordate relationships
A modern lancelet is consequently a comparative relative with its own history, not an unchanged stage through which vertebrates passed. The same warning applies to living hagfish and lampreys. Their anatomy can reveal inherited features and secondary specializations; simplicity alone cannot polarize a character.The New Head hypothesis connects cranial sensory and feeding innovations with neural crest and ectodermal placodes. This is a developmental explanation for assembling a more elaborate head. Experiments on living chordates can test where cells originate, which structures they form and which regulatory interactions are needed. The fossil presence of eyes or branchial supports cannot directly demonstrate the embryonic migration of neural crest. Conversely, a conserved regulatory gene alone does not establish that a complete modern head existed in an Ediacaran ancestor. Developmental, molecular and anatomical evidence address complementary parts of the argument.[ref]
Neural crest and the origin of vertebrates: a new head by Carl Gans and R. Glenn Northcutt. Proposed developmental basis and functional significance of head innovation
Ecological context helps explain why these capacities might diversify. More active swimming, prey detection and food processing can create opportunities and selective pressures for improved sensory and locomotor coordination. molecular oxygen availability constrains the metabolic activities that can be sustained. Erik A. Sperling and colleagues compared modern low-oxygen animal communities and related the scarcity of carnivory at low oxygen levels to hypotheses about Cambrian ecological expansion.[ref]
Oxygen, ecology, and the Cambrian radiation of animals by Erik A. Sperling and others. Modern oxygen-gradient observations and the proposed ecological connection
This motivates a mechanism; environmental correlation alone neither dates the vertebrate ancestor nor establishes oxygenation as a sufficient single cause.The useful conclusion is a constrained historical sequence, with explicit gaps. Ediacaran evidence establishes antecedent animal complexity; Cambrian exceptional preservation documents recognizable early vertebrate combinations; comparative phylogenetics and evolutionary developmental biology test their placement and assembly. molecular clocks can estimate earlier divergences, but their dependence on rates and fossil calibration prevents them from turning every absence into a precise origin date.
A monophyletic group includes an ancestor and all its descendants; a paraphyletic group includes an ancestor but excludes some descendants; a polyphyletic group combines separate lineages while excluding their relevant common ancestry. The distinction concerns how membership relates to a phylogenetic tree, rather than how many visible similarities the members possess.
Consider a simplified tree of living amniotes: mammals form one branch, while the other contains lepidosaurs, turtles and archosaurs; living archosaurs comprise crocodilians and birds. Within the latter branch, birds are surviving dinosaurs. The tree below omits extinct branches and most living diversity, and its branch lengths represent neither age nor quantity of evolutionary change. It illustrates three choices of group on the same ancestry.
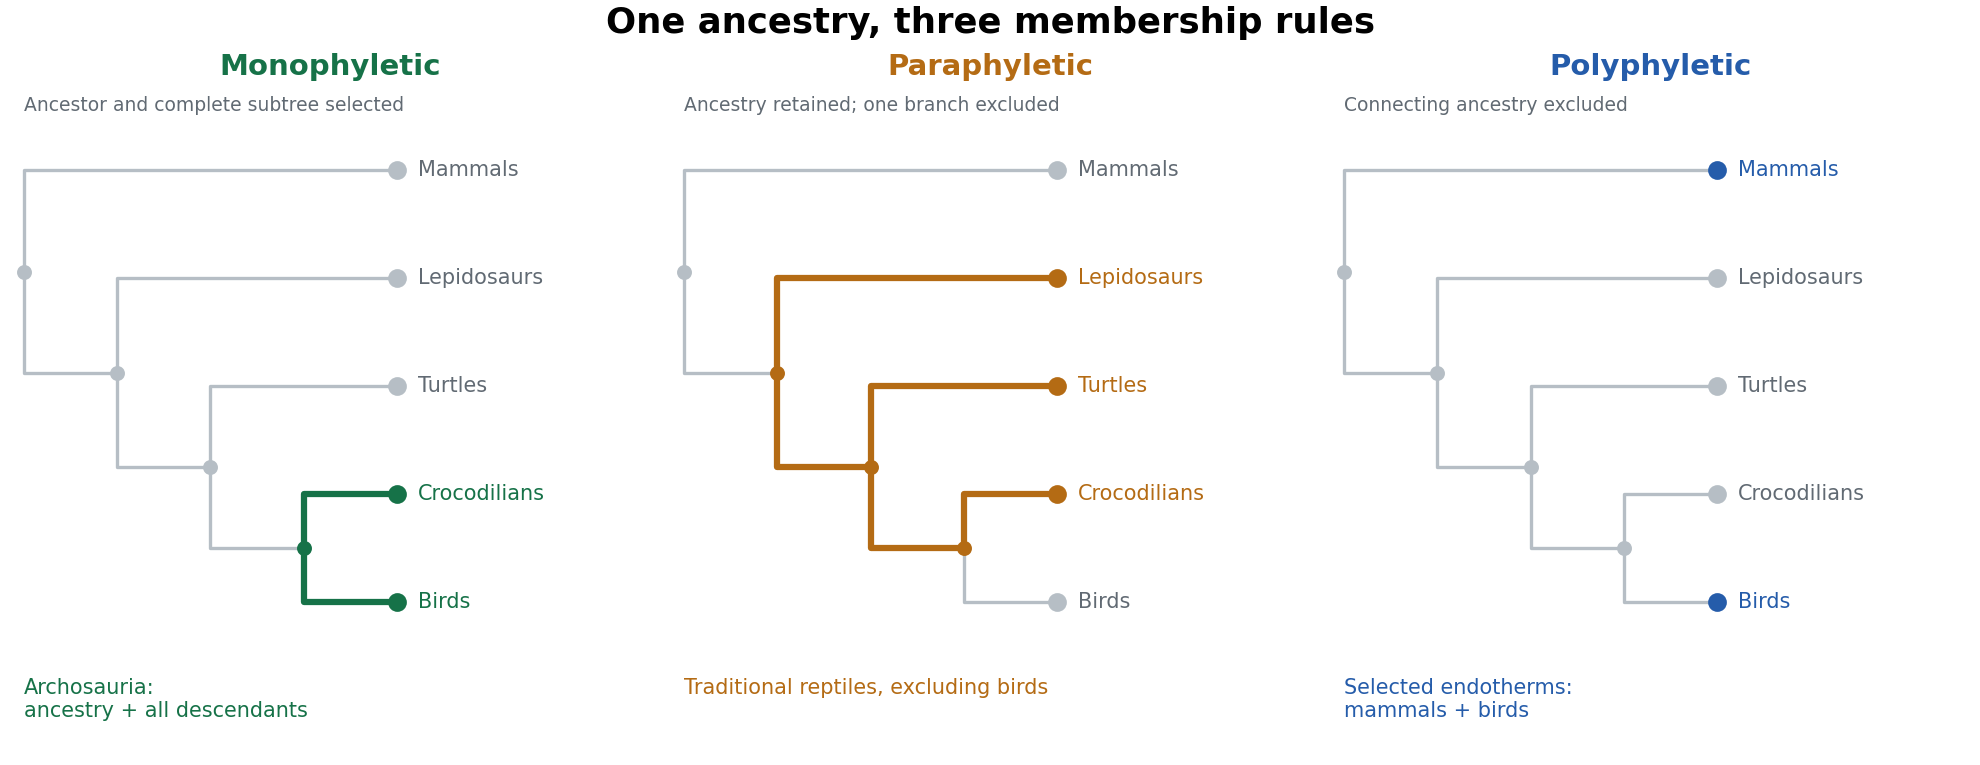

A monophyletic group is a clade. Archosauria includes the last common ancestor of birds and crocodilians and every descendant, including extinct dinosaurs and other extinct branches. In the simplified figure, selecting their shared node and both descendant tips gives the corresponding complete subtree. Sarcopterygii, with tetrapods included, is another example. A clade need not be recognized by a feature that remains visibly unchanged in every descendant: subsequent modification and loss are permitted. It also need not have a particular taxonomic rank.
A familiar paraphyletic group is the traditional assemblage “reptiles” when it includes turtles, lizards, snakes and crocodilians but explicitly excludes birds. The latter descend from within the ancestry otherwise assigned to that assemblage. The selected ancestry is therefore cut short at one of its own branches. Similarly, conventional “fish” that include finned sarcopterygians but exclude tetrapods form an evolutionary grade rather than a complete clade. These examples require the stated usage: Reptilia or Sauropsida can instead be defined as a clade that includes birds. The everyday word does not irrevocably determine the phylogenetic status of every technical definition bearing that name.
For polyphyly, consider assembling mammals and birds solely as the familiar independently evolved examples of sustained high metabolic heat production, while omitting their intervening ancestors and other descendants. This physiological grouping can be useful for comparing endothermy, but it does not identify one exclusive historical lineage. Their last common ancestor also has descendants such as lepidosaurs and crocodilians. On the usual inference of independent elaboration of the relevant physiology, the selected resemblance involves convergent evolution. Calling the assemblage “warm-blooded vertebrates” must not turn a selected physiological trait into evidence that birds are closer to mammals than to crocodilians. Moreover, endothermy and constant body temperature are not identical properties, and living taxon sampling does not locate every thermophysiological transition in extinct lineages.
There is a subtle distinction between the last two cases. A diagram of selected terminal tips alone can show that a group is not a clade, but does not always uniquely distinguish paraphyly from polyphyly. One must state which ancestors are included and the historical interpretation of the defining character. In the orange example, the ancestral reptile lineage is retained and one descendant branch excluded. In the blue example, similar functional outcomes are assembled from separate branches without including the connecting ancestry. The highlighted internal paths in the figure make that difference explicit.
clades are particularly suitable for discussing vertebrate evolution because their nested membership directly expresses common descent. They permit consistent statements such as “birds are dinosaurs” and “humans are sarcopterygians”, while allowing substantial changes in form and function. Shared derived characters, or synapomorphies, provide evidence for branches; shared ancestral states do not uniquely diagnose the smaller groups inheriting them, and independently acquired similarities require separate explanation. This framework makes character transformations testable against a branching history instead of arranging animals in a ladder of increasing complexity.
In practice the phylogenetic tree remains a hypothesis. More characters, better fossils or different evolutionary models can change inferred relationships. Naming a clade with an explicit ancestry-based definition helps keep the statement intelligible when that happens, but does not make the inference immune to error. Anatomical and molecular characters need biological homology assessment, appropriate taxon sampling and uncertainty estimates. For example, genome-scale data and stem-turtle anatomy independently address whether turtles lie near archosaurs, rather than treating one skull condition as sufficient to define the tree.[ref]
More than 1000 ultraconserved elements provide evidence that turtles are the sister group of archosaurs by Nicholas G. Crawford and others. Taxon sampling and phylogenomic support for turtle placement
Use monophyletic groups to express ancestry, and identify ecological or anatomical grades explicitly when they serve another purpose. paraphyletic groups can summarize retained ancestral organization, and polyphyletic groups can support functional comparisons, but neither should silently substitute for a complete lineage.
The avian digit identity frameshift hypothesis proposes that positional condensations conventionally numbered II, III and IV develop morphological identities I, II and III. It separates the place where an anatomical digit develops from the inherited developmental identity expressed there. It is a hypothesis about evolutionary developmental biology, not a frameshift mutation in a DNA reading frame.
The problem arose from comparing two kinds of evidence. The hands of the theropod relatives of birds were traditionally reconstructed as retaining the first three anatomical digits. Their bone relationships and, in appropriate fossils, the phalangeal pattern of two, three and four phalanges supported identities I, II and III. Embryological studies of the bird wing instead assigned the principal surviving condensations to positions II, III and IV within a pentadactyl reference pattern, partly from their relation to the primary skeletal axis. If positional number necessarily fixed morphological identity, the interpretations appeared inconsistent.
biological homology is a historical claim, however, and a developmental coordinate need not be eternally coupled to the same character identity. Günter P. Wagner and Jacques A. Gauthier proposed an evolutionary change in that coupling: an anatomical digit formed at position II could execute an identity-I developmental program, and the two posterior anatomical digits could undergo the corresponding changes.[ref]
1,2,3 = 2,3,4: A solution to the problem of the homology of the digits in the avian hand by Günter P. Wagner and Jacques A. Gauthier. The developmental frameshift proposal reconciling positional and morphological assignments
With denoting a positional condensation and its resulting identity, the classical proposal is:This notation describes a change in specification. It does not mean that a fully formed thumb physically migrated into another anatomical digit's position during development.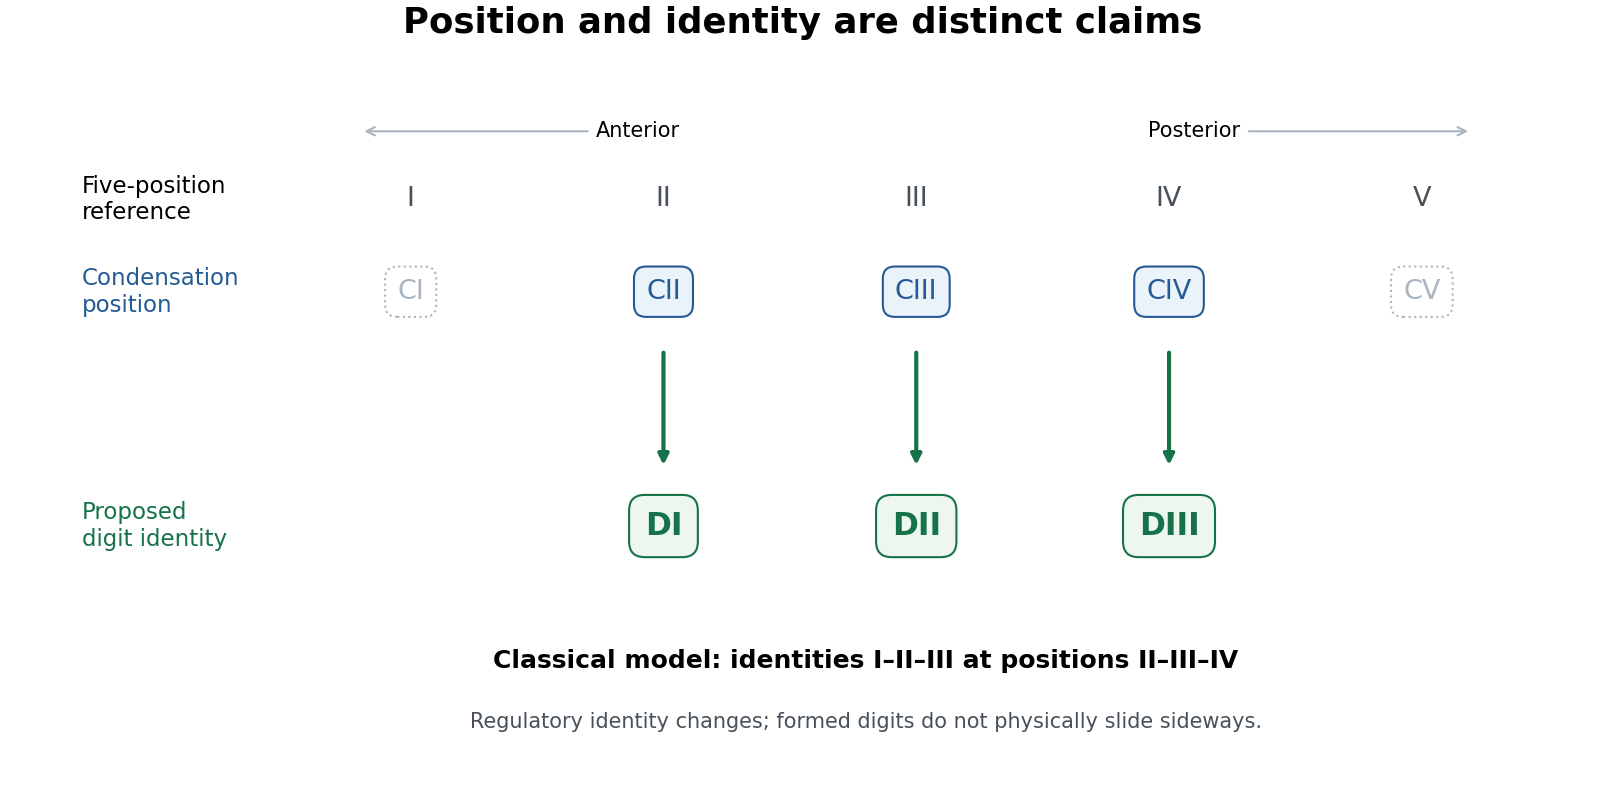
Positional condensations and morphological identities in the classical avian digit frameshift hypothesis
. Original conceptual diagram. The upper row is a five-position reference; the lower rows distinguish the retained positional assignments from the identities proposed for them. Dotted symbols indicate positions outside the three principal retained digits, without asserting that no transient cells or condensations ever occur there. This diagram states the classical model, not a universal molecular identity code. Details.
The proposal yields tests. Anatomical identity should be assessed from several features of metacarpals, joints and phalanges, not by calling the anteriormost remaining anatomical digit “I” by definition. Condensation position should be established independently from staged embryos and fate mapping, rather than inferred solely from the adult hand. Molecular comparisons can then ask whether positional anatomical digit II in the wing shares a distinctive regulatory state with anatomical digit I in a reference limb. evolution of gene regulation, including the duration and distribution of Sonic hedgehog signalling and downstream interactions, offers a means of uncoupling position and later differentiation. Expression of one Hox gene is informative but is not a universally valid barcode of a complete digit identity.
Koji Tamura and colleagues used cell labelling and transplantation to compare wing and hindlimb development. The cells contributing to the posterior wing anatomical digit did not have the same relationship to the posterior signalling region, the zone of polarizing activity, as the corresponding hindlimb anatomical digit IV; their early separation was compatible with a digit-III developmental domain. This supplied experimental evidence against equating the posterior wing anatomical digit straightforwardly with hindlimb anatomical digit IV.[ref]
Embryological evidence identifies wing digits in birds as digits 1, 2, and 3 by Koji Tamura and others. Cell-labelling and transplantation comparisons of wing and hindlimb digit progenitors
Such experiments need embryos matched by developmental stage, verified label positions, assessment of label persistence and spread, and controls for effects of grafting on survival and growth. A cell's ultimate contribution establishes its fate under the tested conditions; it does not alone establish the evolutionary identity of every structure it forms. Comparing forelimb with hindlimb also requires recognizing that the two are already developmentally different organs. The stronger inference combines lineage tracing with anatomy and regulatory evidence.
Transcriptomic data sharpened, rather than simply ended, the debate. Zhe Wang and colleagues found a conserved anterior-digit signature consistent with identity I in the anteriormost wing anatomical digit, while the posterior wing anatomical digits showed derived expression identities rather than a simple conserved series.[ref]
Transcriptomic analysis of avian digits reveals conserved and derived digit identities in birds by Zhe Wang and others. Comparative digit transcriptomes and the distinctive anterior-wing-digit signature
A later multi-species comparison by Thomas A. Stewart and colleagues challenged the assumption that all corresponding anatomical digits possess a conserved tetrapod-wide molecular identity. Their results supported a more limited shift rather than treating every posterior anatomical digit as an unchanged identity displaced by one position.[ref]Evidence against tetrapod-wide digit identities and for a limited frame shift in bird wings by Thomas A. Stewart and others. Cross-species expression comparisons and limits of a universal digit-identity model
Tissue composition, sampling stage, orthology assignment and the choice of reference species are therefore essential controls in molecular tests.The evolutionary significance is substantial but bounded. birds are nested within theropod dinosaurs on evidence extending beyond anatomical digit number, including many skeletal transformations and feathered relatives. The preserved integument of Yutyrannus, for example, documents filamentous feathers in a nonavian tyrannosauroid, broadening the fossil distribution of feathers beyond birds.[ref]
A gigantic feathered dinosaur from the Lower Cretaceous of China by Xing Xu and others. Associated skeletons and filamentous feather preservation in Yutyrannus
A coherent developmental mechanism removes one apparent contradiction between embryology and that historical interpretation. It also illustrates why disagreement between positional and morphological evidence should trigger a mechanistic test rather than automatic rejection of either dataset. However, showing that a regulatory shift is developmentally possible is not proof that precisely the full classical shift occurred in the ancestral bird lineage.The durable result is that anatomical digit position and digit identity can evolve partly independently. Evidence for an identity-I anterior wing anatomical digit is stronger than a claim that all three anatomical digits retain invariant molecular identities I, II and III. The digit identity frameshift hypothesis remains a useful, testable bridge between fossil anatomy and development, with the exact extent and sequence of identity transformation requiring explicit comparison rather than assumed equivalence.
The turtle problem is the difficulty of placing turtles on the reptile phylogenetic tree, historically intensified by conflict between their unusual skulls and other anatomical or molecular evidence. Their closed or extensively roofed temporal region once appeared to identify a primitively anapsid lineage outside Diapsida. Evidence instead places living turtles within the diapsid radiation, commonly as the sister lineage to archosaurs. The inference requires distinguishing retention of an ancestral state from secondary modification.
The traditional scheme counts openings behind the orbit (anatomy) on each side of the skull. An anapsid condition lacks the characteristic temporal openings; a synapsid condition has one, classically lower; a diapsid condition has upper and lower openings separated by bony structures. These descriptions originally provided convenient anatomical categories. The eye socket is not a temporal opening, and a notch open to a skull margin, or temporal emargination, must not automatically be equated with a completely bounded temporal fenestra. bone identities and contacts matter as much as the count.
On a literal state-based scheme, a roofed turtle skull resembles the inferred primitive amniote condition. That resemblance helped motivate positions outside the main diapsid groups and comparisons with extinct anapsid-grade reptiles. Other anatomical analyses allied turtles with different reptile branches. Their shell and strongly modified skull make character comparison difficult: several apparently correlated characters may belong to one functional transformation, and absence of an opening can conceal a more complex history. A shared absence is especially weak evidence when the opening can be closed independently.
Molecular evidence provides an independent character system. Nicholas G. Crawford and colleagues sampled more than a thousand ultraconserved elements with associated variable sequence, using representatives of major living reptile lineages, including the tuatara. Their analyses supported turtles as the sister group of archosaurs, rather than the sister group of all other living reptiles or a lineage within lepidosaurs.[ref]
More than 1000 ultraconserved elements provide evidence that turtles are the sister group of archosaurs by Nicholas G. Crawford and others. Nuclear-locus sampling, inclusion of tuatara and inferred turtle–archosaur relationship
In this hypothesis, crocodilians and birds are closer to one another than either is to turtles. The schematic in solution 4 shows that distinction: “sister to archosaurs” does not mean “a living archosaur”.A large number of aligned bases is not a substitute for checking the analysis. Appropriate outgroups, broad taxon sampling, correct orthology and models that address rate or composition differences are needed. Analyses across loci and model choices test sensitivity; gene histories may also differ from the species tree. Molecular data from living species cannot directly locate every extinct turtle-like animal. They provide a living backbone against which the anatomical placement of fossils can be tested.
Stem-turtle discoveries provide a particularly discriminating anatomical test. Pappochelys, a Middle Triassic animal described by Rainer R. Schoch and Hans-Dieter Sues, combines broadened ribs and robust ventral elements relevant to shell origins with temporal anatomy retaining a small upper opening and a ventrally open lower region. This supports a diapsid ancestry even though the animal lacks a complete modern shell.[ref]
A Middle Triassic stem-turtle and the evolution of the turtle body plan by Rainer R. Schoch and Hans-Dieter Sues. Skull openings, ribs, gastralia and phylogenetic interpretation of Pappochelys
Its significance is the associated character combination, not merely a hole selected because it agrees with a molecular tree. It shows that the shell and temporal roof need not have evolved as one indivisible package.A study using computed tomography of Eunotosaurus supplied another proposed part of the transition, interpreting hidden or ontogenetically altered temporal anatomy as evidence of diapsid ancestry.[ref]
Evolutionary origin of the turtle skull by G. S. Bever and others. Computed-tomographic anatomy, ontogenetic interpretation and placement of Eunotosaurus
The proposed placement of such early forms and the biological homology of particular openings remain matters for character analysis. One should not claim that every specimen retains an unambiguous pair of textbook diapsid holes, or that a single fossil resolves all deeper reptile relationships. Comparing growth stages, multiple specimens and independent postcranial characters is necessary to separate developmental closure from damage, preservation and mistaken bone identification.The general limitation is homoplasy. Openings can expand, merge with a margin, lose separating bars or become secondarily roofed; apparently similar counts can consequently have different histories. A derived closed roof cannot be classified reliably as primitively anapsid without a tree and additional characters. Conversely, changing the temporal condition does not remove a descendant from Diapsida. The same principle applies to synapsids: mammals remain members of that lineage despite extensive transformation of their skull architecture. An anatomical grade is not automatically a clade.
Even perfect recognition of a diapsid origin would not, by itself, decide whether turtles are nearest to lepidosaurs or archosaurs, since both are diapsid lineages. Resolving that question requires informative derived characters within the radiation, rather than recounting the ancestral pair of openings. Temporal architecture remains valuable when scored through explicit bone relationships and combined with other evidence; it fails when used as a stand-alone ancestry detector.
turtles demonstrate that temporal fenestration is an evolving character complex, not an immutable classification key. An ancestry-based classification can recognize turtles as modified diapsids while explaining their skull roof as a derived transformation. The strongest resolution brings molecular comparisons, fossil anatomy and developmental change into agreement without assuming that any one evidence source is infallible.
Patrik L. Ståhl Created 2026-10-20 Updated 2026-11-05
Coauthor of the original spatial-transcriptomics study. The work connected expression measurements from tissue sections with their spatial organization, enabling molecular variation to be compared with tissue anatomy.[ref]
Pectoral girdle Created 2026-10-20 Updated 2026-11-05
The pectoral girdle supports the anterior paired appendages and connects them with the trunk. In humans, the scapula and clavicle provide a mobile arrangement for the upper limb. Comparative anatomy asks which components and connections are shared among vertebrate lineages.
Penis Created 2026-10-31 Updated 2026-11-05
The penis is an external organ containing the terminal urethra and erectile tissue. In human anatomy it participates in urinary outflow and reproductive delivery. Its vascular erectile mechanism is distinct from the neural and muscular coordination of ejaculation.
Perineal body Created 2026-10-31 Updated 2026-11-05
The perineal body is a fibromuscular junction in the perineum where several muscle and connective-tissue elements meet. In female anatomy it lies between the vagina and anal canal. Its value as a support point follows from the convergence of attachments, rather than from being a separate large muscle.
Peter DeSaix Created 2026-10-13 Updated 2026-11-05
Coauthor of Anatomy and Physiology 2e by J. Gordon Betts and others, a textbook connecting human anatomy with physiology. Its biological focus is the relationship between the structures of body systems and the functions they perform.[ref]
Anatomy and Physiology 2e by J. Gordon Betts and others. Verified author or editor credit
Philip D. Gingerich Created 2026-10-20 Updated 2026-11-05
Phylogenetics Created 2026-10-06 Updated 2026-11-05
Phylogenetics infers evolutionary relationships from evidence such as anatomy and DNA sequences. A phylogenetic tree summarizes a proposed pattern of ancestry; phylogenetic characters supply the observations, and an inference procedure states how alternative trees are compared.
For sequence data, a nucleotide substitution model assigns probabilities to changes along branches. The phylogenetic pruning algorithm efficiently sums over unknown ancestral states to compute a likelihood function. This connects a historical hypothesis to an explicit calculation rather than treating the most visually similar species as automatically closest relatives.[ref]
Evolutionary trees from DNA sequences: a maximum likelihood approach by Joseph Felsenstein. Ancestral-state summation and likelihood recursion
Physician Created 2026-10-24 Updated 2026-11-05
A physician is a medically trained professional who investigates and manages human disease and disorders of function. Medical reasoning connects a person's history and examination findings to explanations of altered anatomy and physiology, while comparing alternative causes rather than treating one symptom as a diagnosis.
Pierolapithecus Created 2026-10-20 Updated 2026-11-05
A Miocene fossil ape with a mosaic of trunk and hand characters. Its informative anatomy does not uniquely identify it as the Pan–Homo last common ancestor. [ref]
Pierolapithecus catalaunicus, a new Middle Miocene great ape from Spain by Salvador Moyà-Solà and others. Science 306, pp. 1339–1344; orthograde trunk and contrasting hand morphology