Endosymbiosis is an ecological association in which one organism, the endosymbiont, lives inside another. The definition specifies location, not that both partners benefit, nor that the internal partner has become an organelle. An intracellular association can remain an association between distinct organisms. Endosymbiotic theory addresses a different question: how particular ancestral bacteria became inherited, functionally integrated organelles during evolution.
The striking consequence is that a eukaryotic biological cell can combine histories: its nuclear lineage and its mitochondria need not have the same ancestry. Mitochondria have bacterial ancestry related to Alphaproteobacteria; the plastids of plants and many algae, including chloroplasts, have ancestry within cyanobacteria. These are ancestral lineages, not a claim that a named living bacterial species is the literal ancestor. Present-day bacteria and organelles have both evolved since their shared ancestors. [ref]
Origin and Evolution of Plastids and Photosynthesis in Eukaryotes by Geoffrey I. McFadden. Opening paragraphs and “The endosymbiont: when and who?”: bacterial origins and uncertainty about closest relatives
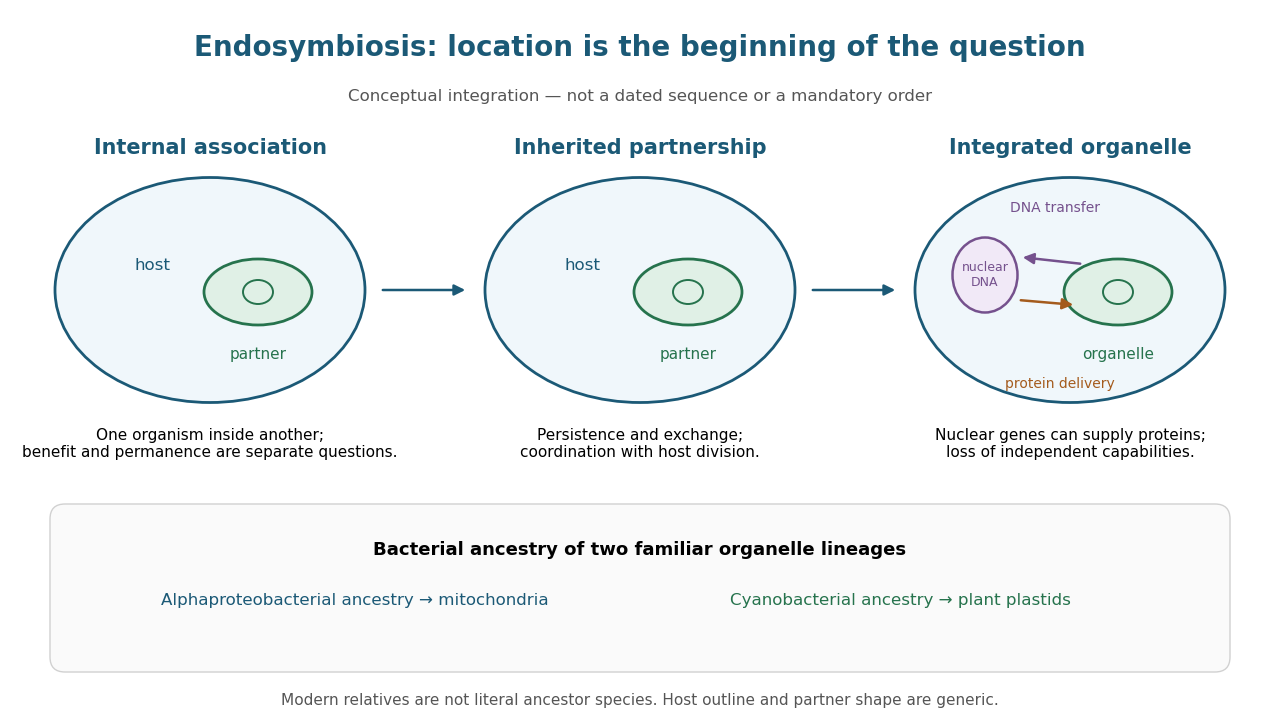
From an internal partner to an integrated organelle
. Original conceptual schematic, not an observed historical sequence. Persistence, metabolic exchange, endosymbiotic gene transfer, organelle protein import and coordination of division illustrate integration; they are not dated stages in a compulsory order. The illustrated partner is generic, and the host outline does not specify the ancestral host of mitochondria. The protein-delivery arrow abbreviates nuclear gene expression, biological translation in the cytosol and organelle protein import; it does not place protein synthesis inside the cell nucleus. Details.
An endosymbiont is the internal partner in an endosymbiosis. Calling an organism an endosymbiont does not by itself classify it as an organelle or imply an irreversible evolutionary transition.
Endosymbiotic theory explains the bacterial origins of mitochondria and plastids through enduring internal associations and subsequent integration. Survival inside a biological cell is only part of the problem: exchange through membrane transport, inherited division, gene expression and delivery of required proteins must work together. The elegance is evolutionary reuse of an existing cellular capability, followed by changes that make the partners operate as one system. [ref]
Origin and Evolution of Plastids and Photosynthesis in Eukaryotes by Geoffrey I. McFadden. Abstract and “How to tame your symbiont”: metabolic, genetic and division integration
The historical On the origin of mitosing cells by Lynn Sagan (1967, abstract and Introduction, pp. 225–226) synthesized a symbiotic account of eukaryotic origins and proposed tests using molecular evidence. Its Introduction explicitly acknowledged earlier proposals. It also hypothesized origins for other structures; the modern evidence for mitochondria and plastids should be assessed separately from the rest of that historical scheme.
Resemblance is a clue, not sufficient evidence of common descent. A small size, two surrounding membranes, division, retained DNA or bacterial-looking ribosomes does not uniquely identify an ancestor. Internal membranes exist outside these organelles, and a similar function can favor similar structures. The stronger question is whether independently examined molecular characters support the same historical relationship.
A concrete genomic observation is the mitochondrial sequence reported in 1997 for Reclinomonas americana: base pairs containing 97 identified genes, including four for a bacterial-type multisubunit RNA polymerase. This is a reported genome inventory, not a calculation from the pictured shape of a mitochondrion. Retention of such bacterial features strengthens the ancestry argument; a living Reclinomonas americana is not itself an ancestral eukaryote. The inspected abstract supplies these observations but not the detailed sequencing protocol or contamination controls, so those details are not attributed to this report here. [ref]
An ancestral mitochondrial DNA resembling a eubacterial genome in miniature by B. Franz Lang and others. Abstract, Nature 387 (1997), pp. 493–497: genome length, gene inventory and bacterial-type RNA polymerase
A sequence-based investigation obtains nucleotide sequences by DNA sequencing, identifies comparable genes, makes a sequence alignment and uses phylogenetics to infer relationships. The readout is a proposed relationship with support and uncertainty, not a photograph of an ancient encounter. Comparisons of plastid sequences with bacterial sequences support cyanobacterial ancestry, while the exact closest sampled cyanobacterial group has depended on the chosen data and inference. A bacterial affinity in one gene is weaker than coherent evidence across several genes and cellular systems. [ref]
Origin and Evolution of Plastids and Photosynthesis in Eukaryotes by Geoffrey I. McFadden. “The endosymbiont: when and who?”: alternative phylogenetic placements and lateral gene transfer
For such an analysis, useful checks include distinguishing organelle DNA from bacterial contamination, verifying sequence quality, comparing corresponding rather than unrelated genes, sampling several bacterial groups and testing sensitivity to the sequence alignment and evolutionary mathematical model. These are methodological requirements, not a claim that this article has rerun a particular published analysis. Horizontal gene transfer, gene loss and unequal evolutionary change can make an individual gene's history differ from a whole organism's history. A supported bacterial origin therefore need not identify an extant donor species, an exact date or the original mode of entry. [ref]
Origin and Evolution of Plastids and Photosynthesis in Eukaryotes by Geoffrey I. McFadden. “The endosymbiont: when and who?”: ancient origin and confounding lateral transfer
Endosymbiotic gene transfer moves genetic material from an endosymbiont or its descendant organelle into the host genome, notably the nuclear genome. A transferred DNA segment can remain silent. For a transferred gene to replace an organelle-encoded function, nuclear gene expression must work and its protein must reach the right compartment through organelle protein import. Transfer of DNA and transport of proteins are distinct processes in opposite directions. [ref]
Experimental Reconstruction of Functional Gene Transfer from the Tobacco Plastid Genome to the Nucleus by Sandra Stegemann and Ralph Bock. Introduction, p. 2869, and Discussion, p. 2875: transferred sequences and the additional targeting problem
Gene loss and endosymbiotic gene transfer are different: absence from an organelle genome does not by itself show that a functional nuclear copy exists. Conversely, an imported protein may derive from a host gene rather than a transferred gene. The surviving organelle genome is therefore a partial record, not a complete inventory of either ancestral bacteria or the modern organelle's machinery. [ref]
Origin and Evolution of Plastids and Photosynthesis in Eukaryotes by Geoffrey I. McFadden. “How to tame your symbiont”: losses, transfers, host recruitment and repatriation of proteins
Experimental Reconstruction of Functional Gene Transfer from the Tobacco Plastid Genome to the Nucleus by Sandra Stegemann and Ralph Bock (2006, Results, pp. 2870–2874) separated relocation of DNA from activation of a relocated gene. Engineered tobacco chloroplasts carried an nptII gene with nuclear expression signals beside an aadA gene with plastid expression signals. Selection on kanamycin recovered plants with the segment in the nuclear genome. Crosses then replaced the engineered chloroplasts with ordinary chloroplasts: the nuclear segment remained, but the plants were initially sensitive to spectinomycin and streptomycin. The transferred aadA gene was not yet functional in its new setting.
Leaf pieces were cultured on regeneration medium containing both drugs. Resistant regenerated plants supplied the functional readout. Using both drugs reduced selection of spontaneous plastid mutations conferring resistance mainly to one drug. Reciprocal crosses and selfing distinguished maternal plastid inheritance from nuclear Mendelian segregation; eight of sixteen initial candidates had the latter pattern. [ref]
Experimental Reconstruction of Functional Gene Transfer from the Tobacco Plastid Genome to the Nucleus by Sandra Stegemann and Ralph Bock. Figure 1, Tables 1–2 and Results, pp. 2870–2871: selection, eliminated candidates and inheritance controls
The molecular readout came from RNA hybridization and DNA sequencing. A Northern blot detected aadA messenger RNA in activated lines, with different transcript sizes. Thermal asymmetric interlaced polymerase chain reaction recovered upstream DNA; products present in activated lines but absent in original-line and ordinary-plant controls were sequenced. The mapped rearrangements connected aadA to the upstream nuclear gene promoter. Thus resistance, inheritance, RNA detection and changed nucleotide sequences supported activation of the transferred nuclear gene, rather than resistance alone. [ref]
Experimental Reconstruction of Functional Gene Transfer from the Tobacco Plastid Genome to the Nucleus by Sandra Stegemann and Ralph Bock. Figures 3–4, Results, pp. 2872–2874, and “PCR and DNA sequencing”/“TAIL-PCR”, pp. 2876–2877
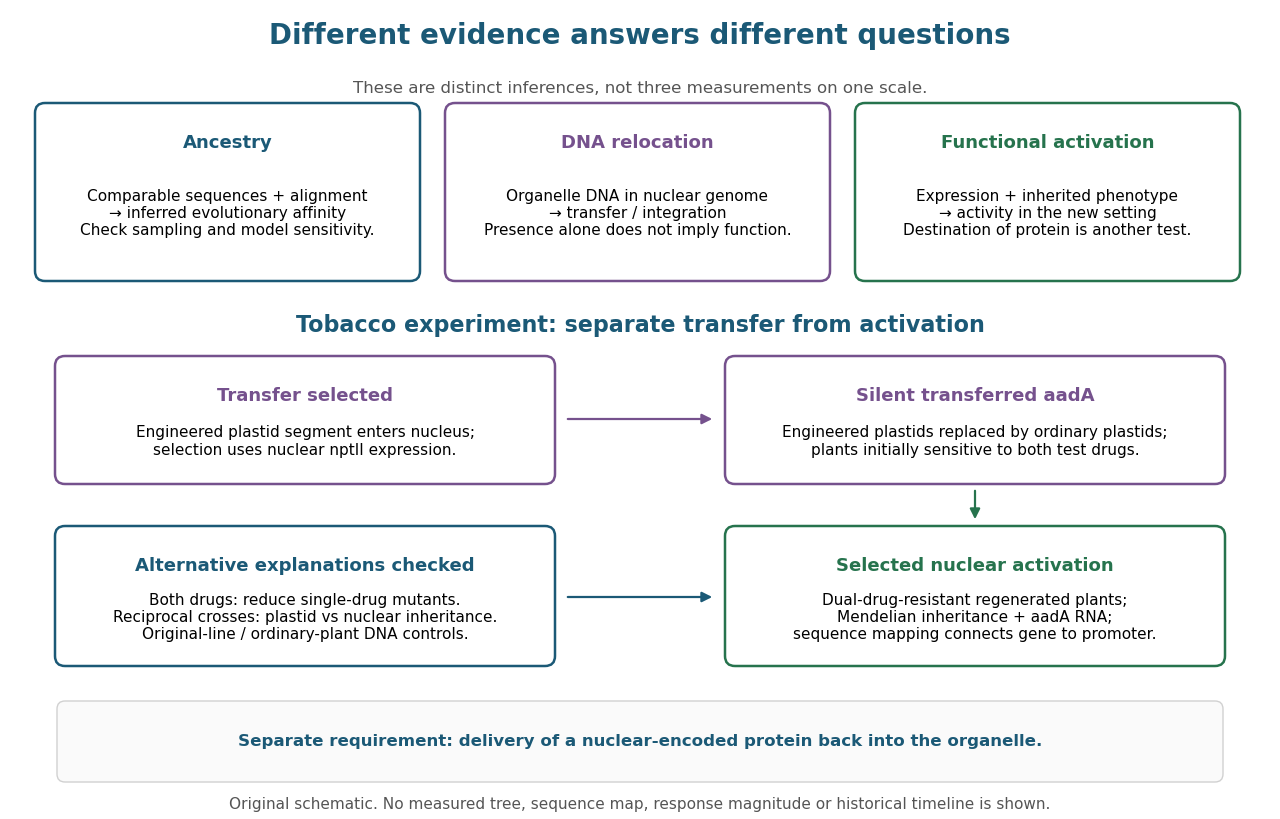

This engineered test demonstrates one route to functional nuclear gene expression after plastid DNA transfer. It does not establish a natural transfer rate, replay ancient endosymbiosis or demonstrate that the resulting protein is imported into a chloroplast. The authors explicitly identify acquisition of targeting information as an additional step not reproduced by this experiment. [ref]
Experimental Reconstruction of Functional Gene Transfer from the Tobacco Plastid Genome to the Nucleus by Sandra Stegemann and Ralph Bock. Discussion, p. 2875: antibiotic selection and missing transit-peptide acquisition
Articles by others on the same topic
There are currently no matching articles.