
Correlative and causal approaches answer different questions, and neither is dispensable for understanding neuromodulation. An intervention is generally stronger evidence about the consequence of changing a specified target, while observation is essential for discovering the naturally occurring signal, its heterogeneity and the contexts in which it appears. Usefulness depends on the claim, measurement and assumptions, not simply on whether an experiment uses an optogenetic actuator.
A correlation between a neuromodulatory signal and behaviour can arise because the signal influences the behaviour, behaviour changes the signal, or a third variable influences both. Reward expectation, movement and arousal often covary. Temporal precedence helps reject some accounts but does not eliminate an unmeasured common cause. Detailed task manipulations can nevertheless make correlative evidence much more discriminating: varying expectation while holding delivered outcome constant tests a different hypothesis from merely comparing rewarded and unrewarded trials.
The dopamine prediction-error account illustrates this value. Patterns across unexpected rewards, predictive cues and omitted expected rewards constrained an explicit computational hypothesis. A generic rise in activity at a reward would not distinguish reward receipt, expectation and error. Recording before intervening helped identify the timing and task conditions in which a putative teaching signal should be manipulated. Without that information, a stimulation experiment might show that a pathway can change behaviour while leaving the proposed natural computation largely unspecified.
Observations also reveal what population averages hide. Cell-resolved dopamine imaging showed structured sensory, motor and cognitive heterogeneity during a navigation task. Comparing identified dopamine spiking with accumbens release revealed that evolving release dynamics need not mirror recorded somatic activity. These findings constrain the target and measurement level of subsequent interventions. They are not failures of observation: a perturbation of an entire heterogeneous population could obscure precisely the functional distinctions that recording discovers.[ref]
Specialized coding of sensory, motor and cognitive variables in VTA dopamine neurons by Ben Engelhard and others. Abstract and cell-resolved encoding analyses: heterogeneous task-variable relationships
[ref]Dissociable dopamine dynamics for learning and motivation by Ali Mohebi and others. Abstract and Figures 2–5: cell-body spiking versus local release
Interventions can then test a well-specified causal prediction. Reward-timed activation of dopamine neurons overcame associative blocking, changing subsequent cue learning; brief inhibition supported a negative-error-like learning effect. These manipulations are stronger evidence for a teaching contribution than a correlation alone. Yet the manipulated population and timing must match the proposed endogenous signal, and later unstimulated testing is needed to separate acquired learning from immediate performance effects. Sufficiency to impose an effect is not proof that the artificial activity pattern occurs naturally or is the only possible teaching route.[ref]
A causal link between prediction errors, dopamine neurons and learning by Elizabeth E. Steinberg and others. Abstract and Figures 1–4: temporally targeted manipulation and subsequent associative learning
[ref]Brief optogenetic inhibition of dopamine neurons mimics endogenous negative reward prediction errors by Chun Yun Chang and others. Abstract and Results: brief inhibition and later learning effects
Claims of functional necessity and sufficiency are conditional. Selective inhibition that impairs performance can support necessity under the tested conditions, but may act through sensation, movement or motivation rather than the hypothesized computation. A null effect can reflect redundant circuits, incomplete target engagement or compensation. Conversely, stimulation can recruit an unnatural synchrony, reverse-propagating activity or multiple collateral targets. Changing neurons identified by one transmitter can also change co-transmission, so the intervention is not automatically selective for that chemical signal at one synapse.
Pharmacological perturbations make similar assumptions visible. A systemic drug affects receptors according to exposure and selectivity, not according to the experimenter’s functional label. Time of testing, peripheral actions, active metabolites and off-target drug effects matter. The chemogenetic ligand clozapine-N-oxide provides a concrete example: receptor-binding and distribution work showed that conversion to clozapine can account for central DREADD activation. Thus an apparent designer-receptor intervention cannot be assumed to have the intended pharmacological isolation merely because the receptor was genetically targeted. Ligand-only controls and exposure measurements improve the causal interpretation.[ref]
Measurement is therefore required inside causal experiments as well as before them. Histology can confirm targeting but not the actual moment-to-moment physiological effect; electrophysiology or transmitter measurements can test target engagement. Calcium signals, fibre photometry, voltammetry and spikes have different spatial, temporal and chemical limitations. Converging methods are more persuasive when they agree at their common resolution, while disagreements can identify local regulation or a mistaken measurement model rather than simply experimental failure.
Causal mediation is a further step. Randomizing a drug can establish an effect of the assigned treatment, but correlating a post-treatment neural signal with symptom change does not prove that signal mediated the effect. Both may reflect another drug consequence. Likewise, statistically controlling for movement can remove a confound in one causal model but remove a genuine intermediate mechanism in another. A causal diagram and an explicit target estimand should guide adjustment rather than a rule to regress out every variable associated with behaviour.
Human and animal approaches have complementary scope. Fine cellular interventions can provide internal validity in a restricted animal task, while human longitudinal observations can test whether candidate abnormalities precede illness and whether the same behavioural dimensions matter clinically. Ethical and practical constraints preclude arbitrary human lesions or perfectly selective transmitter manipulation. It would be unhelpful to discard clinically relevant observation for failing to perform an impossible experiment; equally, a prospective association should not be relabelled as a proven biological cause.
The most productive programme iterates among formal models, naturalistic measurements and selective perturbations. Specify the computation, identify its predicted signal, vary task factors that distinguish alternatives, and intervene with appropriate timing, targeting and performance controls. Re-test the resulting behavioural and neural predictions across contexts. Causal experiments generally have an advantage for a precise intervention question, but correlative approaches remain essential for deciding what should be changed and what the causal result actually explains.
The SOP model family specifies testable principles of stimulus processing and association, but it does not yet have a uniquely established neural implementation. Its behavioural breadth should be distinguished from evidence identifying the biological counterparts of its states, transition rules and separate response systems. The strongest neurobiology concerns processes that the models require—priming, associative retrieval and differentiated response pathways—rather than a one-to-one mapping of every symbol onto a brain structure.
Ivan Pavlov’s classical conditioning tradition made stimulus history and the measured conditioned response objects of controlled experiment. The SOP model introduced by Allan R. Wagner represents stimuli as elements distributed among inactivity , primary activation and secondary activation . External presentation promotes inactive elements into ; activity then passes through before returning to inactivity. A learned associate can activate an expected event directly into . Recently or associatively activated elements are less available for renewed primary processing, distinguishing self-generated priming from retrieval-generated priming. A contemporary quantitative analysis shows how these dynamics can generate several habituation regularities; these are simulations, not measurements of neuronal states.[ref]
A quantitative account of the behavioral characteristics of habituation: the sometimes opponent processes model of stimulus processing by Yerco E. Uribe-Bahamonde and others. The SOP Model section: state occupancy, decay and two sources of priming
The association rules make the account more specific than a generic fading trace. In the original formulation, concurrent and activity promotes excitation, whereas with promotes inhibition. The Modified SOP model additionally permits learning involving a cue activated into : matched-state combinations can strengthen excitation and mismatched-state combinations inhibition. This allows an absent cue’s association to change through retrieval, addressing retrospective revaluation. The model is therefore not simply equivalent to a reward-error equation or to synaptic fatigue.
Human causal-judgment experiments motivated an important constraint. Participants learned relations among compound cues and an outcome, then received information about a companion cue without the target. Retrospective changes in judgments depended on the consistency of earlier within-compound pairings. This supports a role for learned cue–cue relations in revaluation, but the behavioural result does not identify synapses implementing the modified state-pair rules. Other retrieval or inference models can also use knowledge of those relations.[ref]
Within compound associations mediate the retrospective revaluation of causality judgements by Anthony Dickinson and others. Abstract and experiments, pp. 60–80: consistent versus varied compounds and backward revaluation
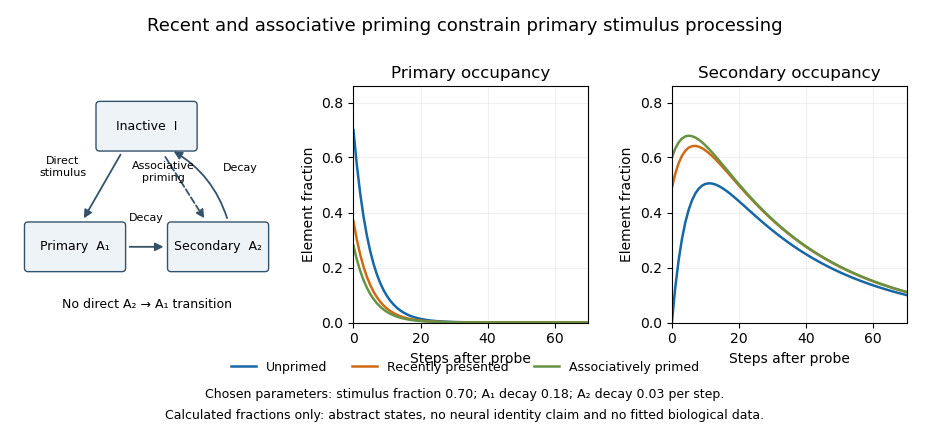
Primary and secondary activation in an original illustrative SOP-style state model
. Calculated occupancy fractions with chosen parameters, not neuronal activity. A recent presentation or associative priming leaves fewer inactive elements available for a subsequent primary response. The figure illustrates the state logic and conservation of probability, not a full SOP, M-SOP or AESOP learning simulation. Details.Neural adaptation alone is insufficient to explain retrieval-generated effects. A transient reduction in response to a repeated physical stimulus could result from receptor adaptation, local synaptic dynamics or wider circuit changes, whereas context-specific long-term priming requires an account of the context’s learned relation to the event. A biological test must distinguish an unfamiliar stimulus from an unexpected combination of familiar stimuli and control attention, orienting and stimulus exposure. Reduced firing cannot simply be labelled : the theory permits secondary activity to be behaviourally silent or have a response-system-dependent effect.
Hippocampal lesion experiments provide evidence at that process level. Rats learned audiovisual sequences in which particular sounds preceded particular lights. Switching the familiar sound–light combinations renewed visual orienting in controls but not in hippocampal-lesioned animals, despite relatively preserved habituation to visual stimuli and evidence of sequence associations. This implicates the hippocampus in associative mismatch rather than novelty alone. It is compatible with a contribution to expectation or retrieval, but does not uniquely show that the hippocampus is , nor that every SOP model process is hippocampal.[ref]
Hippocampal lesions disrupt an associative mismatch process by Robert C. Honey and others. Abstract and pp. 2226–2230: audiovisual sequence switching, orienting and lesion controls
Receptor perturbation further separates short- and long-term components. Mice lacking the GluA1 AMPA-receptor subunit showed impaired short-term spatial novelty performance but enhanced long-term performance under the tested interval conditions. Manipulating exposure and test intervals helped distinguish rapid recency-dependent effects from longer-lasting learning. This is consistent with separable processes of the kind emphasized by the SOP model, rather than an undifferentiated stronger-versus-weaker memory. Nevertheless, a lifelong mutation can alter development and network function, and task dependence prevents identifying GluA1 with a single abstract transition parameter.[ref]
Enhanced long-term and impaired short-term spatial memory in GluA1 AMPA receptor subunit knockout mice: evidence for a dual-process memory model by David J. Sanderson and others. Abstract and Experiments 1–2: exposure/test intervals, spatial novelty and the opposite short-/long-term effects
Associative access to an absent outcome has additional circuit support. In rat sensory preconditioning, orbitofrontal inactivation impaired behaviour guided by an indirectly inferred outcome while sparing behaviour supported by the directly reward-paired cue. The manipulation also altered learning when inferred value normally acted as a blocker. This shows that retrieved associative structure can influence both performance and new learning. It is relevant to the demands of Modified SOP model, but does not demonstrate that the neural representation is in exactly or that its plasticity has the model’s stipulated sign.[ref]
Orbitofrontal cortex supports behavior and learning using inferred but not cached values by Joshua L. Jones and others. Abstract and Figures 1–2: inferred versus directly trained values and reversible inactivation
The Affective extension of SOP, developed by Allan R. Wagner and Susan E. Brandon, distinguishes sensory-specific and emotive components with different processing time courses and response consequences. Behavioural experiments in rabbits showed modulation of a discrete conditioned eyeblink by another putatively emotive conditioned stimulus. Such dissociations motivate separate response components. They do not locate a complete emotive representation in one nucleus. Basic conditioned-eyelid experiments independently implicated cerebellar nuclear circuitry through lesions, recordings and stimulation, illustrating why a motor conditioned response cannot simply be assigned to the same mechanism as every autonomic or emotional effect.[ref]
Modulation of a discrete Pavlovian conditioned reflex by a putative emotive Pavlovian conditioned stimulus by Susan E. Brandon and others. Abstract and pp. 299–311: modulation of the discrete conditioned reflex
[ref]Cerebellum: essential involvement in the classically conditioned eyelid response by David A. McCormick and others. Abstract and pp. 296–299: cerebellar lesions, activity and stimulation
The remaining challenge is discriminative implementation. A candidate neural model should specify what an element is, how direct and retrieved activity differ, how relevant overlap controls plasticity, and how sensory and affective components affect separate outputs. Manipulating receptor function or recording reactivation is not enough unless alternative mechanisms make different predictions. Neuromodulators could regulate transition rates, representation selection or plasticity, but there is no justified general identity such as “dopamine is ” or “serotonin is .” Multiple biological mechanisms could realize the same functional state description.
The SOP model family is therefore a valuable framework connecting stimulus history, expectation and response organization. Primary lesion, receptor and inactivation evidence supports several component processes. Its comprehensive behavioural ambitions exceed what is currently established about its precise neurobiology; the next useful experiments distinguish direct activation from retrieved activation and test the associated plasticity rules, rather than merely find a neural correlate of one familiar behavioural effect.
Reward prediction error remains a strong account of particular phasic dopamine signals and their contribution to learning; it is inadequate as a universal description of every dopamine neuron, projection and timescale. The question is best answered by separating the computational hypothesis, measurements of naturally occurring activity, and evidence that manipulating an error-like signal changes later learning.
In temporal-difference learning, a prediction is updated usingwhere is the value function for state , is the next reward, discounts later return, and is the update step size. The terminal value is zero. A reward prediction error is therefore not simply reward, pleasure or salience. Its sign depends on what was expected and when. An unexpected reward can generate a positive error; an accurately predicted reward can generate little error; omission of an expected reward can generate a negative error. A cue can produce an error when it changes the prediction of future return even though no immediate reward is delivered.
Primate recordings motivated this account because phasic responses changed with learning and reward expectation rather than responding identically to every reward. Linking these patterns to a quantitative learning rule provided predictions about cue responses and outcome omissions that a generic “reward neuron” label lacked. However, extracellular identification and population sampling matter, and the computational state representation is an assumption. A model fitted with a poor description of what the animal knows can misclassify a genuine expectation-related response as a theoretical failure.[ref]
A neural substrate of prediction and reward by Wolfram Schultz and others. Abstract and pp. 1593–1599: linkage between dopaminergic activity, changing predictions and computational learning
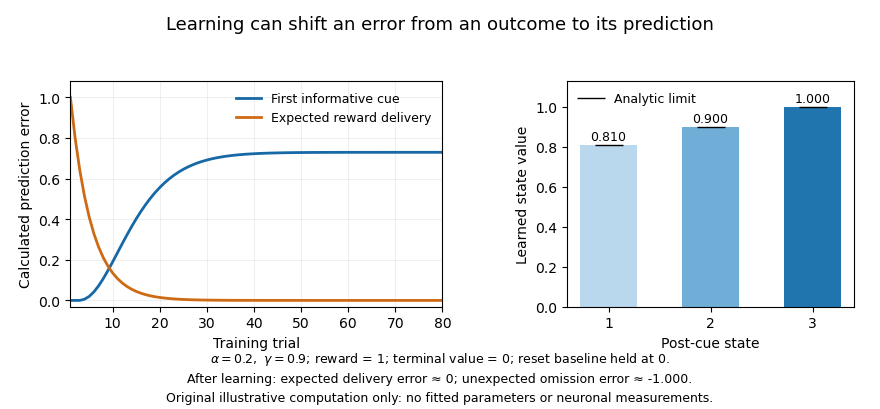
Prediction errors in an original toy temporal-difference learning task
. Calculated learning curves and value estimates for a deterministic state chain; these are not neuronal recordings. A reset trial state supplies the first informative cue. After learning, an unexpected reward omission produces a negative error at the expected reward transition. Details.Association-learning experiments make the interpretation more than a curve-fitting exercise. In blocking, an established cue already predicts the reward, reducing learning about an added cue. Reward-timed optogenetic activation of dopamine neurons could overcome this blocking, supplying an error-like teaching event despite the normally expected reward. The relevant endpoint was subsequent learning about a cue, not just movement during stimulation. This supports a causal teaching contribution but does not establish that artificially synchronized activation reproduces every feature of an endogenous code.[ref]
The negative side of the error also has intervention evidence. Brief inhibition of targeted dopamine neurons around reward processing produced later learning changes resembling those expected from a negative error, with behavioural controls addressing distraction or immediate aversion. This strengthens a bidirectional teaching account beyond sufficiency of excitation alone. The imposed pause still tests a particular population and task, and inhibition can affect processes other than the proposed scalar signal. Appropriate timing controls and later unstimulated testing are essential to the interpretation.[ref]
Brief optogenetic inhibition of dopamine neurons mimics endogenous negative reward prediction errors by Chun Yun Chang and others. Abstract and Results, pp. 111–116: brief inhibition and later associative responding
Population heterogeneity can refine the hypothesis rather than simply refute it. Distributional reinforcement-learning work proposed multiple channels differing in optimism and in their relative sensitivity to positive and negative errors. Mouse single-unit data showed systematic variation in response reversal points consistent with this account. One reward can then be better than expected for one channel and worse for another. The finding challenges a single shared scalar prediction broadcast identically by all cells, while retaining prediction-error-like computations. It does not make heterogeneity alone proof of a particular distributional algorithm.[ref]
A distributional code for value in dopamine-based reinforcement learning by Will Dabney and others. Abstract and Figures 1–5: differential reversal points and distributional predictions
Other heterogeneity is not readily summarized as reward error. Cell-resolved imaging during a mouse virtual-navigation task found dopamine-neuron signals related to sensory, motor and cognitive variables, with structured differences across neurons. Regression and task design can separate some predictors, but correlated movements and expectations limit unique interpretation. Such findings make a universal scalar account implausible; they do not eliminate the well-controlled reward-error results in other populations. Nor should every movement-related signal be re-labelled as error without an independently specified model that predicts it.[ref]
Specialized coding of sensory, motor and cognitive variables in VTA dopamine neurons by Ben Engelhard and others. Abstract and encoding analyses, pp. 509–513: cell-resolved task-variable heterogeneity
The measurement compartment is another limitation. A comparison of identified VTA cell spiking with nucleus-accumbens dopamine release in a common decision task found release dynamics related to evolving reward expectations without corresponding changes in recorded cell-body spiking. Local release regulation therefore matters: a terminal sensor and a somatic spike train need not report the same quantity. This is especially important for interpreting slower ramps or motivational effects as direct readings of a broadcast phasic error.[ref]
Dissociable dopamine dynamics for learning and motivation by Ali Mohebi and others. Abstract and Figures 2–5: comparison of identified spiking and accumbens release dynamics
Further qualifications concern learning itself. An error depends on subjective reward, inferred state, uncertainty and task structure; it is not calculated from the experimenter’s reward schedule alone. Values informed by a model of the environment can also contribute, so identifying an error-like signal does not automatically prove exclusively model-free learning. Conversely, a very flexible state model can accommodate almost any observation unless its representation and parameters are constrained independently. Good tests manipulate expectation while matching outcome and movement, and compare explicit alternatives on held-out behaviour and neural data.
The account is thus still appropriate when stated at the right resolution: some temporally precise dopamine activity supplies expectation-dependent teaching signals, supported by both recordings and causal learning manipulations. A complete account of the dopamine system must additionally explain projection-specific coding, local transmitter dynamics, motivation and movement. The productive revision is a family of constrained computational and circuit hypotheses, rather than either one molecule–one number or abandonment of prediction error altogether.
Non-human experiments have made serotonin’s role in emotion more specific: its effects depend on receptor subtype, developmental history, projection and behavioural demand. Their strength is controlled intervention at levels inaccessible in ordinary human research. Their weakness is that an experimentally altered behaviour is an operational measure, not a direct reading of human emotional experience or an entire psychiatric disorder.
Serotonin arises from heterogeneous neuronal populations and acts through multiple serotonin receptors. Manipulating synthesis, reuptake, a receptor or one projection is not interchangeable. Systemic drug administration can affect many targets, while a permanent depletion permits adaptation. Conversely, temporally restricted intervention can reveal when a pathway matters but imposes a pattern that may differ from natural activity. These distinctions make converging approaches more informative than assigning a single emotional function to the molecule.
Developmental rescue experiments demonstrate why timing matters. Mice lacking 5-HT1A receptors showed increased anxiety-like behaviour; conditional receptor expression largely in hippocampal and cortical targets rescued the measured phenotype when present during an early postnatal period, whereas adult expression alone did not provide the same rescue. This supports a developmental contribution and warns against equating a lifelong genetic perturbation with acute adult treatment. However, rescue establishes sufficiency of the introduced expression pattern under those conditions, not necessarily the endogenous receptor location’s unique necessity. Ectopic expression, altered circuitry and compensatory development remain relevant limitations.[ref]
Serotonin1A receptor acts during development to establish normal anxiety-like behaviour in the adult by Cornelius Gross and others. Abstract and pp. 396–400: conditional spatial and developmental rescue
Local depletion in primates provides a different kind of evidence. Marmosets with prefrontal serotonin depletion perseverated on a previously rewarded visual stimulus when its contingency reversed, while retention of a previously learned discrimination and acquisition of a new one were relatively spared. These controls constrain explanations based on general inability to learn or recognize the stimuli. The result links serotonin to flexible use of changed outcomes, a process relevant to emotion regulation. Yet reversal learning is not itself a measure of sadness, fear or subjective affect, and depletion is not equivalent to an isolated physiological fluctuation.[ref]
Cognitive inflexibility after prefrontal serotonin depletion by Hannah F. Clarke and others. Abstract and pp. 878–880: serial reversals, retention and new-discrimination controls
Optogenetic studies add temporal precision. In mice waiting for delayed rewards, timed activation of dorsal-raphe serotonergic neurons reduced premature abandonment of waiting, including on omission trials. Control experiments argued against simple motor inhibition and against the effect being merely reinforcing. This challenges an account of serotonin as only a punishment or generalized behavioural-inhibition signal. The appropriate conclusion is that activating the targeted population can promote waiting in that task; patience is still a behavioural construct, and the imposed activity does not by itself identify the natural signal’s full content.[ref]
Optogenetic activation of dorsal raphe serotonin neurons enhances patience for future rewards by Kayoko W. Miyazaki and others. Abstract and Results, pp. 2033–2040: delayed-reward waiting and motor/reinforcement controls
A pathway-specific experiment gives the complementary result. Activating serotonergic projections from the dorsal raphe nucleus to the BNST promoted selected anxiety- and fear-related behaviours. Combined anatomical, electrophysiological and pharmacological evidence implicated a local 5-HT2C receptor-sensitive circuit involving corticotropin-releasing hormone neurons. Thus raising serotonergic activity in one pathway can have a different behavioural consequence from activating another population during reward waiting. Local inhibition and disinhibition matter: transmitter effects on one cell class need not have the same sign as the pathway’s net behavioural effect.[ref]
These examples also show how apparatus shapes the claim. Open-arm exploration measures approach–avoidance under environmental threat; conditioned freezing measures one defensive output; visual choice tasks measure outcome-guided flexibility; a reward port allows measurement of waiting and leaving. Each permits careful timing and quantitative controls, but none is a complete emotional state. Converging measures of movement, feeding, autonomic state, discrimination and learned response reduce the risk of interpreting every changed score as an emotional effect.
Species comparisons are informative when they isolate conserved functions rather than presume identical experience. Primates allow some translational similarities in prefrontal organization and complex behaviour; rodents allow larger experimental samples and finer cellular access. Strain, sex, age, housing and prior stress can influence measured phenotypes. Highly controlled laboratory conditions improve internal validity while limiting the contexts over which the result is known to generalize. Inbred animals and one aversive task cannot represent the full diversity of human affective illness.
Cell specificity creates further opportunities and limits. Targeting neurons by a serotonergic marker improves on identifying them only from spike shape or location. Nevertheless, cell populations can differ in projections and co-transmission; stimulating a cell can affect more than serotonin at one target. Terminal stimulation can recruit network or collateral effects, and a receptor antagonist can have off-target drug effects. Claims about a particular released transmitter are stronger when supported by release measurements, receptor-level tests and independent perturbations, not genetic targeting alone.
Temporal comparisons are equally important. Developmental effects concern how a circuit is established; acute effects concern its current operation; repeated pharmacological exposure may change receptor regulation and experience-dependent learning. A behavioural rescue in a genetically altered mouse therefore cannot be read as a prescription for an adult human. Nor does a transient anxiogenic effect contradict every beneficial effect of longer treatment: different times, targets and readouts are being compared.
The best use of animal work is an iterative programme. Specify a computation or response, establish a selective circuit or receptor contribution, test alternative performance explanations, and then examine corresponding predictions with human behavioural and pharmacological measures. Animal experiments have already replaced a simple “more serotonin means better mood” story with mechanistic heterogeneity. Their translational value increases when they identify that heterogeneity and its boundary conditions rather than claim that one manipulation models all emotion.
Learning and memory provide powerful mechanistic accounts of some psychiatric symptoms, but they are not an adequate single-level definition of all psychiatric disorders. The most useful claim is that abnormal learning, valuation or retrieval can mediate particular symptoms and interact with biological vulnerability and environment. Calling every persistent symptom a “memory” without specifying a computation, mechanism and discriminating prediction would make the account unfalsifiable.
Several causal positions must be separated. A learning abnormality could precede illness and increase vulnerability, mediate the expression of an established biological disturbance, or follow from the illness, medication or adverse experiences. A cross-sectional task deficit does not distinguish these possibilities. Nor does a diagnosis identify one latent parameter: poor performance can result from altered motivation, perception, attention, beliefs or motor output as well as learning. Construct validity and external validity are therefore central, not afterthoughts.
For schizophrenia, an influential proposal links dopamine dysregulation to aberrant salience. Events or internal representations acquire inappropriate significance, and attempts to explain those experiences can contribute to delusions. This creates a possible bridge between neurochemistry and acquired belief. It is a theoretical framework rather than evidence that each psychotic belief is an ordinary reinforced association; psychosis is also not specific to schizophrenia. The account must explain which symptoms it predicts and which remain outside its scope.[ref]
Psychosis as a state of aberrant salience: a framework linking biology, phenomenology, and pharmacology in schizophrenia by Shitij Kapur. Abstract and pp. 13–23: proposed salience framework and its stated explanatory scope
A pharmacological experiment provides a more direct test of one link. Healthy volunteers performed causal associative learning during randomized ketamine and placebo sessions with functional magnetic resonance imaging. The drug perturbed right-frontal responses related to violated expectations, and individual neural responses were related to subsequently assessed perceptual and belief-like drug effects. This supports an association between altered learning-related processing and psychotomimetic experience. It does not show that ketamine reproduces the developmental course of schizophrenia, or that the observed imaging signal is the unique mediator of a delusion. Pharmacology causally changes the drug condition; the relationship between an imaging response and a symptom remains a separate inferential step.[ref]
Frontal responses during learning predict vulnerability to the psychotogenic effects of ketamine: linking cognition, brain activity, and psychosis by Philip R. Corlett and others. Abstract; Results and Comment, pp. 611–621: randomized drug challenge, learning responses and symptom relations
Prospective evidence helps with temporal ordering. Elevated striatal dopamine synthesis capacity was observed before transition to psychotic disorder in a high-risk cohort. That finding is important biological evidence, but a PET synthesis-capacity estimate does not directly measure trial-wise reward prediction errors, and elevated capacity does not establish a specific learning algorithm. It also does not imply that every high-risk person or every diagnosed patient has the same abnormality. A learning account should connect this biological vulnerability to task-defined computations rather than substitute one measure for another.[ref]
Dopamine synthesis capacity before onset of psychosis by Oliver D. Howes and others. Abstract and pp. 1311–1317: prospective imaging and transition-group comparison
For major depressive disorder, low expectations of control, persistent negative interpretations and reduced engagement with rewarding opportunities are plausible learning-related mechanisms. Learned helplessness provides a specific model of how uncontrollability can change later behaviour; attributional style helps explain generalization and persistence in human accounts. These mechanisms are neither a moral judgment about the individual nor proof that all adverse circumstances are controllable. Sleep, bodily symptoms, neurodevelopmental factors and the diversity of depressive presentations remain part of the explanandum.
Behavioural evidence is more precise than a global claim that depressed people “cannot learn.” In a probabilistic reward task, unmedicated depressed participants showed reduced development of response bias toward a more frequently rewarded stimulus, with analyses implicating integration of reinforcement history rather than total absence of response to an individual reward. This separates one aspect of reward learning from subjective pleasure and from every component of anhedonia. The direction of causation remains open in a cross-sectional comparison.[ref]
Treatment findings can also link biological and cognitive levels. An acute norepinephrine-reuptake manipulation changed emotional processing in depressed participants before subjective mood changed. That observation is consistent with pharmacologically altered experience processing contributing to later improvement; it does not prove that the early task change mediates every later clinical response. Learning and pharmacology can interact rather than constitute mutually exclusive treatments. A drug might alter the conditions under which corrective experiences are encoded, while behavioural intervention supplies those experiences.[ref]
Effect of acute antidepressant administration on negative affective bias in depressed patients by Catherine J. Harmer and others. Abstract; Methods and Results: early emotional-processing effects without immediate mood change
The learning perspective generates concrete treatment hypotheses. In threat disorders, extinction learning suggests improving safety learning and its retrieval across contexts, rather than merely suppressing an immediate response. A randomized pilot study combined D-cycloserine or placebo with virtual-reality exposure to heights in people with acrophobia. Greater improvement in the adjunct condition provided an early proof of concept for facilitating a specified learning experience. The small, specific trial does not establish a general cognitive enhancer for all diagnoses, and an intervention that facilitates learning need not selectively strengthen desirable information. Treatment timing and the quality of the learning episode are therefore empirical issues.[ref]
Cognitive enhancers as adjuncts to psychotherapy: use of D-cycloserine in phobic individuals to facilitate extinction of fear by Kerry J. Ressler and others. Abstract and pp. 1136–1144: blinded randomized pilot, virtual glass-elevator exposure and follow-up
For psychotic symptoms, a learning account predicts that reducing inappropriate salience may permit new interpretation without instantly deleting established beliefs. For depression, it motivates tests of changes in reward sensitivity, information integration and expectations, with functional recovery as an outcome. These are treatment-development hypotheses, not conclusions that a single task parameter should dictate care. Symptom improvement, correction of a proposed mechanism and prevention of relapse require separate measurements; changing a laboratory score is not sufficient evidence of benefit.
The broad claim becomes convincing only when models predict specific patterns, survive controls for performance confounds, and show temporally appropriate changes linked to symptoms. Comparisons with unaffected high-risk individuals, longitudinal designs and mechanism-sensitive randomized trials can distinguish vulnerability, mediation and consequence. Learning and memory are therefore valuable explanatory levels and possible treatment targets, especially for particular acquired responses and beliefs. They do not replace the biological, developmental and social causes of psychiatric illness, and they should not turn diagnostic heterogeneity into one assumed defect.
Fear and anxiety share learning mechanisms, neuromodulators and defensive circuitry, but differ in how threat is specified and sustained. A useful operational distinction is an immediate response to an identified danger versus prolonged anticipation of uncertain danger. That distinction should not be mistaken for a universal division into two independent brain centres. Neuropsychopharmacology is most informative when it compares matched behavioural endpoints and identifies where and when a drug acts.
The first issue is measurement. Freezing, avoidance, autonomic changes, fear-potentiated startle and subjective reports capture different aspects of threat responding. A rat’s reduced open-arm exploration can reflect anxiety, but also altered movement or novelty preference. A smaller startle response can reflect sedation rather than reduced threat processing. It is therefore necessary to measure baseline responsiveness, locomotion and sensory function, and to distinguish acquisition, consolidation, retrieval and expression. A drug administered only at testing does not establish an effect on the original learning.
An influential rat experiment compared potentiation of acoustic startle by a conditioned threat cue with enhancement during sustained bright illumination. Local AMPA receptor antagonism in the central nucleus of the amygdala disrupted the conditioned-cue effect, whereas antagonism in the bed nucleus of the stria terminalis disrupted the light-enhanced effect. The basolateral amygdala contributed to both. This is stronger evidence for differentiation than comparing unrelated assays because the measured reflex was shared. However, conditioning history, stimulus properties and duration differed together, so the result does not isolate duration or uncertainty as the sole cause of the dissociation.[ref]
Double dissociation between the involvement of the bed nucleus of the stria terminalis and the central nucleus of the amygdala in startle increases produced by conditioned versus unconditioned fear by David L. Walker and others. Abstract and Figures 2–5: local glutamate-receptor antagonism and two startle-potentiation paradigms
The amygdala and BNST belong to interacting networks receiving cortical and other inputs and influencing hypothalamic and brainstem outputs. The hippocampus supplies contextual information and prefrontal cortex can influence threat regulation and extinction retrieval. Subdivisions and projection-defined populations within the extended amygdala can differ in function. A general claim that the amygdala produces all fear and the BNST produces all anxiety consequently ignores shared pathways, task dependence and cellular heterogeneity.
Fast inhibitory signalling supplies an important pharmacological comparison. Many benzodiazepines positively modulate susceptible GABA-A receptors, but anxiolysis must be distinguished from sedation and amnesia. A controlled human crossover study compared predictable-cue, unpredictable-threat and no-threat conditions. Alprazolam reduced sustained contextual startle enhancement at the effective tested treatment condition while leaving phasic cue potentiation relatively unaffected. The design included an active sedating comparison as well as placebo. This supports psychopharmacological differentiation between sustained and phasic measures; it does not prove absolute drug selectivity for a subjective state or show that every clinical anxiety presentation has the same mechanism.[ref]
The benzodiazepine alprazolam dissociates contextual fear from cued fear in humans as assessed by fear-potentiated startle by Christian Grillon and others. Abstract and pp. 760–766: crossover treatments, predictable/unpredictable threat and phasic versus sustained startle
Serotonin illustrates why transmitter identity alone is insufficient. Reuptake inhibition affects multiple receptors and projection targets, and early effects can differ from adaptations after repeated treatment. In mice, a dorsal-raphe projection to the BNST recruited a serotonin-sensitive local circuit and promoted selected threat-related behaviours. This provides a pathway-specific explanation for an anxiogenic effect of increasing serotonin signalling, compatible with different effects at other targets. It is not evidence that serotonin uniformly causes anxiety or that rodent threat responses establish the clinical time course of an SSRI.[ref]
Serotonin engages an anxiety and fear-promoting circuit in the extended amygdala by Catherine A. Marcinkiewcz and others. Abstract and Figure 1: dorsal-raphe–BNST projection and threat-related behaviour
Receptor subtype and developmental timing also matter. The same receptor class can act as an autoreceptor controlling raphe output or on non-serotonergic target neurons. Norepinephrine, corticotropin-releasing hormone and other modulators interact with these systems rather than map one-to-one onto fear or anxiety. Local circuit effects should not be inferred from circulating hormone concentrations. A mechanistic explanation should state the receptor, target, timescale and outcome, not merely whether a brain-wide chemical level rose or fell.
Learning about safety supplies both a shared mechanism and a therapeutic distinction. In extinction learning, an expected aversive outcome is omitted; reduced responding can reflect new inhibitory or contextual knowledge rather than deletion of the original association. In rats, the NMDA receptor partial agonist D-cycloserine facilitated later reduction of conditioned startle when combined with extinction training. Its effect depended on learning conditions rather than acting simply as an acute suppressant of every defensive response. This motivates a learning-adjunct strategy, but the animal result alone cannot establish clinical efficacy.[ref]
Facilitation of conditioned fear extinction by systemic administration or intra-amygdala infusions of D-cycloserine as assessed with fear-potentiated startle in rats by David L. Walker and others. Abstract and Results: extinction-dependent facilitation assessed with conditioned startle
Anxiety about uncertain contexts can involve more than a response to one cue: broad threat generalization, avoidance that prevents corrective experience, and context-dependent retrieval may sustain it. Conversely, a sharply defined learned cue can acquire persistent control. Exposure therapy therefore cannot be reduced to suppressing an output on one occasion. An intervention that changes expression without improving subsequent safety learning might have a different long-term effect from one that changes what is retained. Renewal after extinction also predicts that improvement in one context need not transfer automatically to another.
The strongest comparison is thus dimensional and mechanistic. Fear and anxiety share synaptic plasticity, inhibitory signalling and distributed threat networks, while particular temporal and informational demands recruit distinguishable components. Drug and circuit dissociations are meaningful when matched controls rule out motor or sensory explanations; they should refine this network account rather than replace it with a pair of transmitter labels. These are conclusions about evidence and experimental models, not instructions for selecting medication.
Spatial and chemical multisensory processing share problems of binding, uncertainty, learning and common-cause attribution. They often differ in what their inputs represent: spatial cues can estimate the same location, whereas taste and odor frequently supply complementary attributes of a food. The comparison concerns particular computations and tasks, not a rigid separation between two kinds of brain.
In spatial localization, vision, audition and touch can each provide information about position, although they begin in different coordinates. Visual information is initially related to the retina, auditory location depends on binaural and spectral cues, and touch is related to a body surface. Combining them requires accounting for eye, head and body position. Spatial coincidence supports a common event, but is not sufficient: unrelated events can occur nearby, and one moving object can produce cues at different times.
A simple reliability-weighted cue integration model makes a precise prediction. Suppose are unbiased, independent estimates of one position, with variances . An unbiased linear estimate is , withDifferentiating and setting the derivative to zero yieldsThe second derivative is positive. The minimum-variance two-cue estimate assigns greater weight to the more precise cue, and independent information reduces variance below either individual variance. With independent Gaussian noise and a flat prior, minimizing the negative log-likelihood gives the same weighted mean. Correlated errors, bias, a nonflat prior or separate causes change this benchmark.
Marc O. Ernst and Martin S. Banks measured visual and haptic estimates of object height and compared combined judgments with predictions based on unisensory variability. Manipulating visual uncertainty and cue conflict supported reliability-dependent weighting and improved combined precision in that task.[ref]
Humans integrate visual and haptic information in a statistically optimal fashion by Marc O. Ernst and Martin S. Banks. Nature 415, 429–433; apparatus, unisensory estimates and combined-cue predictions
The conclusion is conditional optimality for measured inputs and task, not that every multisensory judgment or neuron always computes an optimum.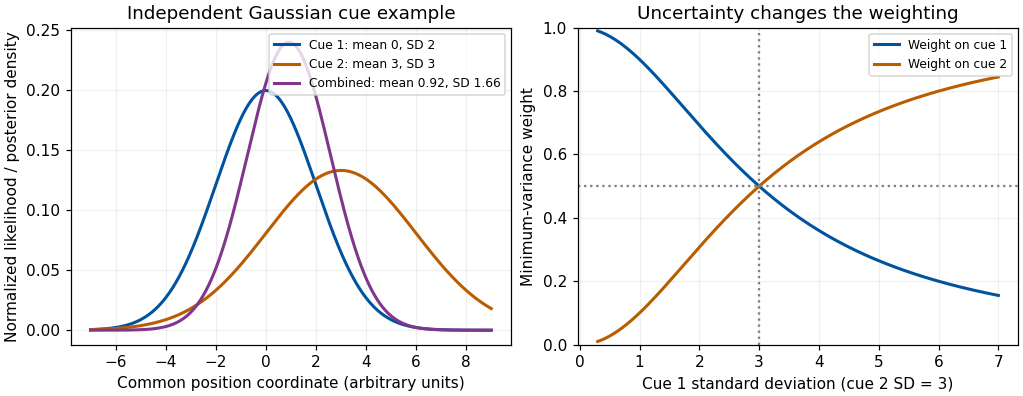
Original independent-Gaussian cue model: likelihood multiplication and variance-minimizing weights; curves are theoretical examples, not experimental results
. Details. Development supplies a useful qualification. Monica Gori and colleagues measured visual, haptic and combined judgments of block size and orientation in children. Younger children did not always obtain the adult-like precision gain; the dominant modality differed between size and orientation, and adult-like combination emerged around eight to ten years in those tests.[ref]
Young children do not integrate visual and haptic form information by Monica Gori and others. Curr Biol 18, 694–698; size and orientation tasks and age comparisons
The authors proposed a role for cross-sensory calibration. The result does not establish one universal maturation age for all multisensory tasks. It shows why adult cue-combination rules should not simply be assigned to every developing observer.The chemical senses pose a different representational problem. Gustation responds to dissolved chemicals at taste receptors, while olfaction responds to volatile molecules; oral touch, temperature and irritation also contribute to a food percept. Retronasal odor can be attributed to the mouth through olfactory referral, even though its receptors remain in the nose. A sweet taste and a fruit odor are not necessarily two noisy measurements of one physical sweetness coordinate. They can jointly identify a food or predict nutritional and hedonic properties. Adding them with inverse-variance weights is therefore not automatically meaningful.
Nevertheless, the same inferential questions arise: do signals belong to the same food, how should prior experience affect interpretation, and which component is responsible for a judged quality? Richard J. Stevenson and colleagues' odor–taste conditioning results show that pairing an odor with sweet or sour tastes can alter later odor judgments.[ref]
The acquisition of taste properties by odors by Richard J. Stevenson and others. Learning and Motivation 26, 433–455; Experiment 1
Learned co-occurrence can thus influence flavor qualities. Verbal confusion or a rating change alone does not establish full sensory fusion; separate taste, odor and pleasantness scales help test response dumping.Neural convergence is also shared without implying identical architectures. Ivan E. T. de Araujo and colleagues delivered tastes and retronasal odors separately and together during human functional magnetic resonance imaging. They identified overlapping responses in several regions and interactions in orbitofrontal cortex; some responses also covaried with consonance or pleasantness ratings.[ref]
Taste-olfactory convergence, and the representation of the pleasantness of flavour, in the human brain by Ivan E. T. de Araujo and others. Eur J Neurosci 18, 2059–2068; event-related taste, retronasal odor and mixture contrasts
A mixture interaction is stronger evidence than overlap alone, but an imaging voxel does not prove that every responding neuron receives both inputs. A neural correlation with pleasantness also differs from a causal explanation of food preference.Temporal and spatial structure further distinguish typical tasks. Spatial audiovisual cues can be brief, externally localized events; food perception unfolds with sniffing, chewing, dissolution and swallowing. Taste and retronasal odor may be bound despite unlike onset profiles because their sequence is expected within eating. Chemical signals can adapt and interact at peripheral as well as central stages, while vision and audition face their own receptor and pathway nonlinearities. Neither class is exclusively early or late, automatic or attention-dependent. Attention, task instructions, hunger and learned expectations can change what is selected or reported; these influences must be measured rather than inferred from a unitary percept alone.
A decisive comparison therefore uses matched inferential questions: estimate a common property, identify a common object, or judge whether two signals share a cause. Measure unisensory performance, test cue conflict and temporal or semantic congruence, and distinguish changes in quality, uncertainty and response. Both domains integrate evidence about events; spatial averaging is a useful special case, while complementary chemical information often requires object, quality and value representations beyond a shared coordinate.
Crossmodal correspondences can guide a sensory-substitution code toward distinctions users can learn and retain, but intuitive mappings do not guarantee useful spatial information or effortless perception. Design must respect both the information supplied by the device and the limitations and goals of the remaining sensory system.
A sensory substitution system captures information normally available through one sensory channel and recodes it for another. A camera-to-sound device does not restore photoreceptors: an auditory listener learns to interpret a controlled relation between image properties and sounds. That differs from multisensory cue integration, where two functioning channels provide estimates of the same event. Residual vision, touch or action can nevertheless interact with the substituted information, so integration and substitution can coexist in actual use.
Historically, Paul Bach-y-Rita and collaborators investigated television-camera information presented through tactile stimulation. Their 1969 report established an early experimental program for tactile image projection as an aid and as a test of sensory processing.[ref]
Vision Substitution by Tactile Image Projection by Paul Bach-y-Rita and others. Nature 221, 963–964; apparatus rationale and early substitution report
This history matters because useful access to object structure need not reproduce the original receptor input. A successful task, however, does not by itself establish that the participant has acquired ordinary visual experience.A concrete engineering example is Peter B. L. Meijer's vOICe. The original system sampled camera images and scanned columns from left to right. Horizontal position became time within the scan, vertical position became tone frequency, and pixel brightness controlled amplitude. A computer-based inverse reconstruction tested preservation of image information in the acoustic code; the 1992 paper explicitly distinguished that engineering result from an established resolution of human perception.[ref]
An experimental system for auditory image representations by Peter B. L. Meijer. IEEE Trans Biomed Eng 39, 112–121; Abstract and Image-to-Sound Mapping
An invertible signal representation can still be difficult for a listener to decode.For illustration, let be brightness at row and column , with row index increasing upward. During column a simple encoder outputsThe scan schedule labels horizontal position; the frequency labels vertical position; labels brightness. Under ideal sampling and orthogonal tones, amplitude extraction recovers the column coefficients. Finite presentation times, masking, frequency resolution and noise limit human recoverability. Increasing the number of pixels can increase transmitted information without increasing usable perceptual detail.
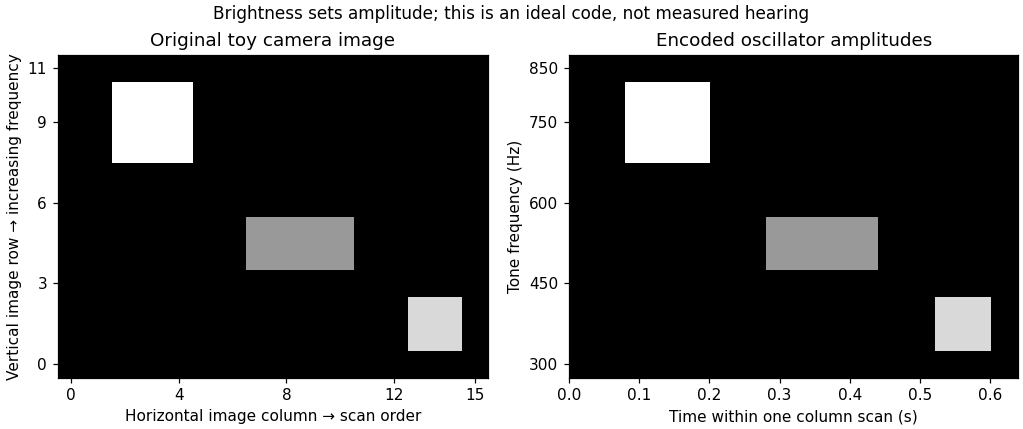
Original toy image-to-sound code: column order becomes scan time, upward position becomes increasing frequency, and brightness sets amplitude; no participant data or copied apparatus figure
. Details. Correspondence knowledge supplies candidate defaults. Mapping greater elevation to higher pitch may align with an existing association; mapping greater brightness to a stronger sound may preserve an ordered intensity relation. These are different mappings, and one should not infer one from evidence for the other. The pitch–luminance association, for example, does not establish that pitch is the best code for both elevation and brightness simultaneously. Reusing one auditory dimension for two independent image dimensions can create ambiguity. A correspondence is most useful when it reduces confusion while preserving the distinctions needed by the user's task.
Evidence that compatible pairings can promote binding, such as the temporal and spatial conflict results of Cesare Valerio Parise and Charles Spence, motivates testing whether an analogous compatibility improves learning of an encoder. It is not a direct comparison of substitution devices. Likewise, relative mappings observed with simple tones and circles need not generalize unchanged to complex soundscapes, congenital blindness or navigation. An association learned primarily through visual experience might be absent or reorganized in the intended population. Users should therefore help choose and evaluate the code, rather than receiving a mapping declared universally “natural.”
Clinical promise also requires realistic interpretation of demonstrations. Ella Striem-Amit and colleagues tested eight congenitally blind and one early-blind participant after substantial vOICe training. Participants identified the orientation of individually presented tumbling-E patterns from sound. Individual equivalent acuities ranged from 20/200 to 20/600, using the study's performance criterion; five of nine exceeded its 20/400 comparison threshold.[ref]
Visual acuity of the congenitally blind using visual-to-auditory sensory substitution by Ella Striem-Amit and others. PLoS ONE 7:e33136; Participants, Experimental design and Results
Those are task-specific visual-pattern judgments through audition, not recovered sight, instant expertise or proof of safe real-world mobility. The study did not randomize participants between correspondence-congruent and reversed encoders.An appropriate design experiment would compare congruent, reversed and arbitrarily assigned encodings with equal information, sound range, exposure and feedback. Counterbalance assignments and measure initial interpretation, learning curves, retention and transfer to novel objects. Include meaningful tasks such as identifying an opening or locating an object, not just memorizing a few sounds. Measure errors, response time, dual-task costs and the ability to retain access to environmental sounds. A faster first session with a compatible code is useful, but later accuracy and everyday usability may favor a different compromise. No outcomes of this proposed experiment are assumed here.
Finally, action can provide calibration. Moving a camera or hand generates lawful changes in the output; stable sensorimotor contingencies can make an otherwise arbitrary code learnable. Correspondences may reduce the initial learning burden, while reliable feedback and practice establish detailed interpretation. Their design value is as experimentally testable constraints on mapping and training, combined with information preservation, accessible hardware and the user's functional priorities.
Practice contributes substantially to compensatory performance after sensory loss, but evidence for selective crossmodal recruitment and causal changes in neural contribution goes beyond an account based solely on accumulated task repetitions. Practice and plasticity are not mutually exclusive: practice can induce neural change, while deprivation can change which circuits practice recruits.
The first requirement is to specify the claimed enhancement. Better tactile discrimination, peripheral visual localization and visual motion detection are different outcomes. Accuracy can improve because of sensory precision, attention, memory, a decision criterion or a slower response. There is no inference from success on one selected task to a universal sharpening of the remaining senses. Sensory loss also differs in onset, completeness, cause and duration. Early blindness, late blindness and temporary blindfolding cannot be treated as equivalent experiments.
A practice account predicts learning with repeated use, specificity to trained inputs and possible transfer to related tasks. A deprivation account predicts changes associated with absent input even when practice is matched. Both can operate, and a statistical difference between groups cannot by itself separate them: daily experience, motivation and selection into a study can differ along with sensory status. Years of Braille use, for example, are not randomly assigned. Comparing blind and sighted experts is more informative than comparing one expert group with novices, but expertise matching does not remove every difference in lifetime experience.
A controlled human study by Lotfi B. Merabet and colleagues used five days of complete blindfolding in normally sighted adults during intensive tactile training, with non-blindfolded training controls. Tactile stimulation increasingly recruited occipital cortex in the deprived group. Disrupting occipital function with repetitive transcranial magnetic stimulation impaired Braille-character discrimination in the blindfolded group on day five, but not in controls; the differential disruption was absent 24 hours after blindfold removal. The imaging response also reversed rapidly.[ref]
Rapid and reversible recruitment of early visual cortex for touch by Lotfi B. Merabet and others. PLoS ONE 3:e3046; Results, TMS results and Discussion
The imaging and stimulation arms used different participants, so one should not claim a within-person correlation between their measures.This combination is more informative than cortical activation alone. Both groups received training, yet the deprived group temporarily depended on a different cortical contribution. Rapid reversibility is compatible with altered weighting or unmasking of existing connections; it does not require wholesale growth of new long-range pathways in five days. The result establishes a functional contribution under the tested state, not that occipital recruitment is sufficient for every tactile gain. Stimulation can affect a network, and the study cannot directly equate sudden reversible deprivation with lifelong blindness. Nor is the persistence of learned skill after the imaging effect disappears paradoxical: skill can remain while the supporting network changes.
A complementary causal result comes from Stephen G. Lomber and colleagues' experiments in congenitally deaf cats. Compared with hearing cats, these animals showed enhanced peripheral visual localization and motion detection on particular tasks. Reversible cooling of posterior auditory cortex removed the localization advantage, whereas cooling a dorsal auditory region removed the motion advantage.[ref]
Cross-modal plasticity in specific auditory cortices underlies visual compensations in the deaf by Stephen G. Lomber and others. Nat Neurosci 13, 1421–1427; visual task battery, reversible deactivation and double dissociation
Cooling provides an experimental contrast between a functioning and temporarily deactivated circuit. The task-specific double dissociation argues for functionally differentiated recruitment, rather than one undifferentiated increase in effort. The evidence is from cats and does not quantify the contribution of practice versus deprivation in humans.A double dissociation is powerful but not magical. To interpret it, one must check that deactivation does not merely impair movement, alertness or basic visibility, and that tasks are not placed at incomparable difficulty levels. The existence of a recruited circuit identifies part of the implementation, not the entire developmental cause. Extensive experience could help establish that circuit's new role. Thus the strict opposition “neural reorganization or practice” confuses a mechanism with one possible source of the mechanism.
A discriminating program would measure performance before training, randomly assign normally sighted participants to matched training with or without temporary deprivation where appropriate, and follow learning and recovery. For established sensory loss, longitudinal observations and carefully matched comparison groups can constrain onset and experience effects without pretending that sensory loss can be freely randomized. Untrained tasks, different body sites or stimulus dimensions, delayed tests and speed–accuracy measurements distinguish broad transfer from repeated response memorization. Peripheral sensitivity should be checked before attributing every difference to cortex. These are design recommendations, not invented completed studies.
Measurement also needs a mechanistic bridge. Fitting psychometric functions can separate threshold and lapse changes; signal detection theory can distinguish sensitivity from a shifted decision criterion under explicit assumptions. Imaging identifies candidate recruitment, while causal disruption tests contribution. Neither activation magnitude nor a lower threshold alone establishes a “better” brain, and an adaptation useful for one task may create costs elsewhere. Residual input, age of onset and the sensory dimension previously calibrated by the missing modality can all constrain outcomes. Enhancement and impairment can coexist in the same person.
The evidence therefore supports an interaction among altered input, experience and circuit availability. Some compensation is task practice, some reflects state-dependent or developmental changes in neural recruitment, and the strongest explanation specifies how those factors cooperate rather than assigning every gain to only one.
Multisensory signals lose synchrony through propagation, receptor and neural delays, and the temporal structure of the event itself. Perceived simultaneity is maintained by tolerance, calibration and inference about common causes, rather than by an infallible clock that makes every channel arrive together. Physical simultaneity, simultaneous receptor stimulation and subjective simultaneity are different quantities.
For an audiovisual event at distance , let auditory and visual propagation speeds be , and processing delays to a specified comparison stage be . A simple internal arrival-time difference, auditory minus visual, isThis follows by subtracting the two sums of travel time and processing delay. At 10 m, using m/s and m/s, the propagation term is about 29.15 ms; at 100 m it is about 291.54 ms. These are calculations under fixed conditions, not perceptual thresholds. Sound speed varies with the medium and temperature. A fixed neural correction could compensate one distance but cannot eliminate propagation differences at every distance.
The neural terms are not fixed constants either. Phototransduction, cochlear transduction, peripheral conduction, stimulus intensity, contrast and the pathway used to define a response can affect latency. A weak or ambiguous stimulus can require more evidence before a decision. Attention, expectations and the selected feature may affect reported timing, without requiring a change in the physical stimulus. A neural onset response, identification response and button press do not mark the same stage. Therefore a reported audiovisual delay should not be casually equated with a single axonal conduction time.
Some apparent desynchronization originates in the source. Lip and jaw movements can precede the acoustic release of speech. A seen hand movement can precede contact and its sound; food handling, oral touch, dissolved tastants and retronasal odor release have different physical time courses. Reverberation can add later auditory energy. Electronic capture, buffering and displays can introduce additional modality-specific delays. The useful goal is consequently to recover whether signals belong to one event and when that event occurred, not to force equal onsets for all its components.
One solution is a temporal binding window: a range of disparities within which signals can be grouped or judged as simultaneous. The window is measured through a specified task, not a universal duration. In a simultaneity judgment, report probability often has a peak around a point of subjective simultaneity. In a temporal order judgment, performance changes from one reported order to the other across offsets. Those measures can differ because their decisions and criteria differ. A broad simultaneity function can reflect uncertain timing or a liberal response criterion; it does not uniquely measure a long neural integration window.
Consider a Gaussian simultaneity decision model. Let physical auditory-minus-visual onset difference be , stable internal offset , and Gaussian timing noise of standard deviation . If the observer reports simultaneous when , thenThe expression is the probability that the noisy difference falls between the two decision bounds. Its center is for symmetric bounds and noise. Increasing makes the observer more tolerant; increasing makes timing less precise. A shift in , a criterion change and extra noise can thus alter different aspects of a measured curve. This is an illustrative model, not a fitted account of the experiment below.
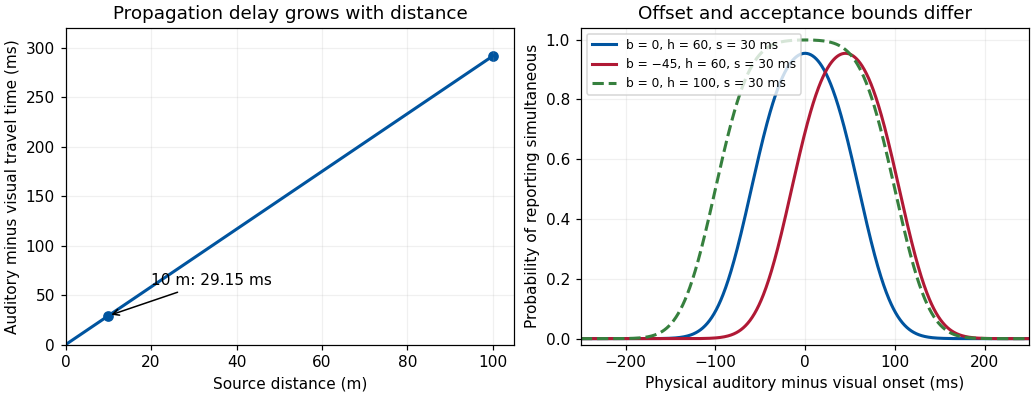
Original propagation calculation and Gaussian simultaneity-decision examples; model parameters are illustrative, not measured temporal binding windows
. Details. Temporal recalibration shows that the offset is adaptable. Waka Fujisaki and colleagues repeatedly paired tone pips and ring flashes at a fixed lag, then measured judgments across test lags. Initial adaptation lasted three minutes with brief re-adaptation before tests. Subjective simultaneity shifted toward the experienced lag; changes in an auditory-induced visual illusion gave evidence beyond a simple change in verbal simultaneity responses.[ref]
Recalibration of audiovisual simultaneity by Waka Fujisaki and others. Nat Neurosci 7, 773–778; Simultaneity judgments and illusion transfer
The adjustment was partial, not exact cancellation of the exposure lag. Transfer constrains a purely task-specific response explanation, but does not locate one unique neural clock or exclude all decision contributions.A complementary strategy is Bayesian causal inference in perception. In a toy Bayesian model, a measured discrepancy has Gaussian variance , while a common-event prior favors discrepancy zero with variance . Completing the square in the product of likelihood and prior proves the Gaussian temporal-discrepancy shrinkage relationThus noisy discrepancies can be pulled toward coincidence. This is a conditional model of one-event inference. A system must also allow separate causes: otherwise a loud unrelated sound would be bound to any nearby flash. Spatial agreement, identity, semantic fit, repeated correlation and action–outcome contingencies can affect that causal judgment. A large discrepancy can lead to segregation rather than endless recalibration.
Calibration and tolerance have costs. A wide acceptance range can stabilize a natural event while merging unrelated events; strong adaptation can help with a delayed device but temporarily bias judgments after it is removed. A convincing experiment therefore controls device timing, intensity and spatial cues, distinguishes order from simultaneity reports, and tests transfer and recovery. Perceptual unity is a flexible estimate supported by delayed and noisy evidence; it preserves useful event structure without guaranteeing veridical timing in every circumstance.
Single-unit recording has been exceptionally fruitful in identifying where and under what conditions multisensory signals interact. Its contribution to human perception is mechanistic and constraining; one cell's discharge is not a complete account of a conscious multisensory event. The strongest conclusions combine cellular recording with behavior, perturbation and models at a comparable computational level.
The essential advance is resolution. An extracellular electrode can isolate action potentials from a neuron, allowing experimenters to map its receptive fields in several sensory modalities, vary stimulus timing and intensity, and compare repeated trials. A cell responsive to light and sound demonstrates convergence at the output of that cell, rather than merely neighboring visual and auditory activity within one imaging voxel. Yet lack of an overt auditory response does not establish lack of auditory input: an input can modulate responsiveness without crossing the cell's firing threshold by itself.
Classic experiments by M. Alex Meredith and Barry E. Stein compared visual, auditory and somatosensory stimuli individually and in combination in the cat superior colliculus. Deep-layer neurons showed enhancement or depression when modalities were combined; many sampled cells had access to descending pathways relevant to orienting.[ref]
Visual, auditory, and somatosensory convergence on cells in superior colliculus results in multisensory integration by M. Alex Meredith and Barry E. Stein. J Neurophysiol 56, 640–662; comparisons of unimodal and combined responses and descending projections
This supplied an experimentally tractable mechanism for using several weak cues to guide an action. It did not require a distinct central place where every sensation becomes conscious.Response enhancement must be defined against an explicit benchmark. Let and be mean stimulus-evoked spike counts after subtracting the matched spontaneous count, and the similarly corrected paired response. Enhancement above the strongest input means . Superadditive multisensory response means the stronger condition . A response can satisfy the former without the latter. Subtracting baseline consistently matters because summing two raw counts also sums spontaneous activity twice. Trial variability and the analysis window determine whether an apparent inequality is statistically credible.
The spatial and temporal rules added testable organization. Mapping stimulus positions relative to each modality's receptive field showed that spatial alignment could favor enhancement, while other arrangements could yield suppression.[ref]
Spatial factors determine the activity of multisensory neurons in cat superior colliculus by M. Alex Meredith and Barry E. Stein. Brain Res 365, 350–354; spatial arrangement relative to receptive fields
Subsequent timing experiments found maximal enhancement when modality-specific peak discharge periods overlapped, with weaker or even depressive interactions at other offsets.[ref]Determinants of multisensory integration in superior colliculus neurons. I. Temporal factors by M. Alex Meredith and others. J Neurosci 7, 3215–3229; response-train overlap and temporal-disparity manipulations
The relevant coincidence is neural, so equal physical onset times need not maximize a cell's interaction.Inverse effectiveness further challenged an account based only on strong signals: the percentage enhancement was often largest when the isolated stimuli evoked weak responses. But the percentage measure itself needs care. If and , enhancement above the strongest response is 300%; if the corresponding values are 20, 20 and 26, it is 30%, although the absolute increment is six in both examples. These invented numbers illustrate a denominator effect, not a measured neuron. Percentage enhancement, absolute gain, information and behavioral benefit are distinct. Weak inputs can give biologically important interactions, but a large ratio alone is not enough to establish special multiplication or perceptual optimality.
Cellular and behavioral definitions of integration also differ. Faster responses to audiovisual than to either unisensory stimuli might arise from a redundant-signals race model: two channels race to trigger a response. If context-invariant channel completion times are , thenThis race model inequality follows from the union bound and does not require independent channels. Violation rejects that race account under its assumptions, but does not identify which collicular or cortical cells produced the effect. Conversely, a nonlinear cell response need not produce a detectable behavioral advantage if other stages limit performance.
Translation to humans requires care about species, sampled structure, task and state. The superior colliculus is well suited to studying orienting, but flavor identity, speech comprehension and deliberate causal judgments need additional circuits. Animal preparation and restraint can change the operating state; a sampled cell population may not represent every multisensory computation. Spiking also reflects recurrent and descending influences, not just a feed-forward meeting of modalities. Human functional magnetic resonance imaging has broader coverage but coactivation cannot establish convergence in one neuron. Timing measures, eye movements, psychophysical cue conflicts and causal perturbations provide complementary constraints.
A useful bridge is to ask whether cellular mechanisms predict a specific human outcome: which weak cue improves localization, which offset permits binding, or when a distractor suppresses orienting. Multisensory cue integration models predict changes in estimates and uncertainty, which are not the same quantity as firing-rate enhancement. Development and learning must also be tested rather than inferred from mature animal responses. Single-cell work supplied fundamental interaction rules and plausible circuit operations; explaining human multisensory experience requires linking those operations to population codes, task-specific decisions and causal behavioral evidence.
Crossmodal correspondences differ meaningfully in what is associated, how the association is acquired and where it affects performance. A matching preference, a response-compatibility effect and altered perceptual binding are distinct observations. They need not have distinct underlying causes, and a single correspondence can have several causes.
A crossmodal correspondence is a systematic relation between attributes in different sensory modalities, such as auditory pitch and visual size. It does not require either stimulus to generate an extra conscious sensation. Thus it should not automatically be classified as developmental synesthesia, where stable inducer–concurrent experiences may be highly individual. Nor is correspondence equivalent to multisensory integration: judging that two attributes fit together does not establish that information from them was combined into one estimate.
Three useful explanatory distinctions concern sensory organization, environmental statistics and meaning. A structural crossmodal correspondence would arise from shared coding or magnitude organization; this predicts a relation surviving changes in labels and response assignments. A statistical crossmodal correspondence would link features repeatedly generated by the same objects. For example, geometrically similar resonators with a fixed wave speed have characteristic frequencies scaling approximately as inverse size: from , increasing lowers . This conditional physical relation can make pitch–size coupling informative, but different materials, tensions or sound-production mechanisms can reverse a simple rule. A semantic crossmodal correspondence can link dimensions through language or common concepts: “high” can describe pitch and elevation. An affective crossmodal correspondence could instead be mediated by shared pleasantness, which should be separated from a direct relation between sensory dimensions. These are explanatory hypotheses, not mutually exclusive boxes established by the appearance of a pairing.
Some correspondences are relative rather than absolute. A tone can be the higher member of one pair and the lower member of another. An experiment should therefore manipulate comparison range and context, rather than assuming that every participant has one fixed pitch-to-size conversion. Relations can also be asymmetric: an irrelevant sound might alter a visual response without a visual stimulus equivalently altering auditory judgment. Asymmetry can arise from task reliability or attention, so it does not by itself establish a one-way anatomical connection.
A comparative experiment provides an important constraint. Vera U. Ludwig and colleagues tested 33 humans and six chimpanzees on matching black and white squares while irrelevant high or low tones were played. Both groups performed better for high-pitch/white and low-pitch/black pairings; in chimpanzees the effect was expressed particularly in errors, whereas human errors were near floor and reaction times were more informative. Both species used a touchscreen and loudspeaker arrangement.[ref]
Visuoauditory mappings between high luminance and high pitch are shared by chimpanzees and humans by Vera U. Ludwig and others. PNAS 108, 20661–20665; Results, Apparatus and Procedure
This makes a human-language-only account inadequate for that mapping. It does not distinguish inherited organization from every form of nonlinguistic learning: the animals had substantial task experience, and shared environments can also generate shared associations.A stronger test of perceptual consequences changes the dependent variable. Cesare Valerio Parise and Charles Spence presented small/large visual stimuli with high/low tones and manipulated audiovisual timing or position. Participants judged temporal order or spatial discrepancy, rather than simply reporting which pairing they preferred. Matched pairings produced poorer access to the intersensory discrepancy, interpreted as stronger coupling.[ref]
When Birds of a Feather Flock Together: Synesthetic Correspondences Modulate Audiovisual Integration in Non-Synesthetes by Cesare Valerio Parise and Charles Spence. PLoS ONE 4:e5664; Experiments 1–3
This illustrates why increased binding need not improve every task: reducing conflict between estimates can make the conflict itself harder to discriminate. A changed discrimination threshold still needs controls for distraction, detectability and decision strategy; it does not uniquely identify a perceptual fusion mechanism.To distinguish mechanisms experimentally, first obtain unisensory detection and discrimination measures and equate unintended salience differences. Then compare explicit matching, speeded classification, conflict discrimination and judgments of a common object. Counterbalance response keys and reverse stimulus–response mappings. A congruency effect that follows the response rule suggests compatibility at a decision or motor stage; persistence under orthogonal response rules constrains that explanation. Fit psychometric functions to conflict judgments and estimate bias, slope and lapses separately. A shift in subjective equality and a loss of sensitivity are different outcomes.
Next manipulate experience. Randomly assign participants to congruent, reversed or uncorrelated audiovisual training with equal exposures, and test untrained exemplars and delayed retention. A reversible mapping with transfer supports an experience-dependent contribution; failure to reverse it does not prove innateness, because training may be weak or poorly measured. Cross-language comparisons with nonverbal responses can test whether a shared word is necessary. Infant or nonhuman results can constrain linguistic explanations, but age differences, task accessibility and species-specific response demands remain possible confounds. For a pleasantness account, collect independent pleasantness ratings and select or manipulate stimuli so that hedonic matching varies separately from the sensory pairing. These are proposed discriminating designs, not asserted experimental results.
The most useful classification therefore combines origin, representational content and measurable consequence. Correspondences are scientifically informative when their predicted transfer, context dependence and effects on sensitivity distinguish them from mere agreement about labels or response keys.
Use the usual empty-coalition normalization for a transferable utility game. Write , so the proposed payoff is the marginal contributionThe vector is the marginal contribution vector for the natural player order.
First, convex cooperative games have increasing marginal contributions. If and , apply the defining supermodular set function inequality to and :Rearranging gives
The vector is efficient by a telescoping sum:Now fix any coalition . For each , its earlier members are . Increasing marginal contributions therefore giveSum over the members of in increasing order. The right-hand side is another telescoping sum, now along the growing coalition :Efficiency and these inequalities for every coalition are exactly the defining requirements of the core of a cooperative game. Thus belongs to the core. The same proof works for any player ordering, not only the natural order.
The normalization is essential to the literal statement: the printed part does not explicitly state it. Without , take the constant characteristic function of a coalitional game . It satisfies the displayed convex cooperative game inequality with equality, but every proposed is zero, so efficiency fails when is nonempty. Under the standard normalized definition, the proof above establishes the intended result.
Let . If the two disjoint winning coalitions exchange players, the aggregate weight is conserved:If both resulting coalitions lost, each weight would be strictly below , making their sum strictly below . This is impossible. Thus every weighted voting game has swap robustness for disjoint winning coalitions, even when the weights or quota are negative.
The converse is false. The four-player prime-cardinality game from part (a) has swap robustness for disjoint winning coalitions: swapping one player each way preserves each coalition's cardinality, so in fact both winning coalitions remain winning. Part (a) proves it is not a weighted voting game.
Even imposing monotonicity would not repair the converse under the printed disjointness restriction. As a stronger counterexample, use five players and declare a coalition winning exactly when it contains player and contains either both or both . This is a simple cooperative game, and all its winning coalitions contain player , so no two are disjoint; the stated swap condition holds vacuously.
Nevertheless and win, while and lose. Both pairs contain every player the same total number of times. A weighted representation would therefore givea contradiction. This is a trade obstruction to weighted voting and pinpoints how weak the disjoint-only swap requirement is.
It suffices to take four players. Both two-player coalitions and win, because two is a prime number, while the empty coalition and the four-player coalition lose.
Suppose real weights and quota represented this game. The empty coalition loses, so . The two winning coalitions requireAdding givesso the four-player coalition must win, a contradiction. Hence prime-cardinality games cannot in general be represented as weighted voting games. The same four-player obstruction appears inside every such game with at least four players.
This proof permits negative individual weights, as the printed definition does. An argument based solely on monotonicity would require a nonnegative-weight assumption and would not suffice for that definition.
This is an absent-minded decision problem: the two decision nodes belong to the same information set. A behavioural strategy must therefore use the same probability at both visits. Put and ; fresh randomization occurs independently at each visit.
The terminal probabilities are for stopping immediately, for going down once and then right, and for going down twice. Thus the expected payoff isThis expression gives the unique global maximum on :
The optimal behavioural strategy improves on either fixed plan
. Details. The independence of repeated randomizations is essential. A mixed strategy choosing once between the two deterministic plans “always ” and “always ” gives at most , since their payoffs are and . It cannot arrange “ first, then ” as a deterministic plan respecting this information set. The failure of perfect recall is exactly why mixed strategies and behavioural strategies need not have the same attainable outcome distributions here.
Measure all payoffs in millions of dollars, in the order (Ann, Bob). Since both players maximize expected money, those numbers are already their expected utility scale.
In the extensive-form game, Ann moves first. Staying out terminates at . Entering leads to Bob's observed decision between fighting, with terminal payoffs , and acquiescing, with terminal payoffs . Each decision node is its own information set, so this is a perfect-information game.


The corresponding normal-form game gives Ann the pure strategies (stay out) and (enter), and Bob the complete contingent pure strategies (fight if entry occurs) and (acquiesce if entry occurs). The payoff matrix isThe pure strategy Nash equilibria are and . Against , Ann prefers ; against , Ann prefers . When Ann stays out, Bob's contingent response does not affect his payoff, so is a best response there.
There is exactly one subgame perfect equilibrium, . In the subgame following entry, Bob strictly prefers to , so backward induction selects acquiescence; Ann then strictly prefers entering for to staying out for . The threat supporting is not optimal in that one-shot subgame.
For infinite repetition, the paper specifies no discount factor. First take the long-run average payoff convention, with all past actions observed. The feasible payoff set is the convex hullAnn can guarantee in every stage by staying out; Bob can guarantee at least in every stage by acquiescing whenever entry occurs. These guarantees are also their minmax payoffs: fighting holds Ann's best possible stage payoff to , and entering holds Bob's best possible stage payoff to .
Therefore the sustainable Nash equilibrium average payoffs are exactly the feasible, weakly individually rational payoffs in a repeated game:This is the closed triangle with vertices .
Here is a direct sufficiency argument for this particular game. Choose a publicly known sequence of stage outcomes whose frequencies give the target point. Before any observed deviation, follow that sequence. After an Ann deviation, Bob fights forever, so Ann can thereafter obtain at most per stage. After a Bob deviation, Ann enters forever, so Bob can thereafter obtain at most per stage. A finite prefix has no effect on long-run average payoff, so no unilateral deviation improves a target with . Rational frequencies can be implemented periodically; arbitrary real frequencies can be implemented by a deterministic sequence with convergent frequencies. Thus even the weak boundary is covered here. In particular, staying out forever and entry followed by acquiescence forever are sustainable; fighting forever is not.
The feasible payoff set and sustainable long-run average payoffs
. Details. 
For discounted payoffs , the folk theorem for repeated games instead gives the usual patience qualification: every feasible point with can be sustained for all sufficiently large . It does not classify the whole region for an unspecified fixed . The two one-shot Nash equilibrium outcomes remain sustainable for every .[ref]
Lecture 15: Repeated Games by Asu Ozdaglar. Slides 19–20 and 24–27: feasibility, minmax bounds, discounted Nash folk theorem and punishment construction
Finally consider the particular history-dependent pair in the paper. Initially Bob has never acquiesced, so Ann stays out. That preserves the same condition forever, giving payoffs . The pair is a Nash equilibrium. Holding Bob's strategy fixed, Ann cannot induce an acquiescence: he fights whenever she enters, and his rule never changes unless he has previously acquiesced. Every entry would give her instead of , so no unilateral deviation helps. Holding Ann's strategy fixed, Bob never reaches a decision node because she stays out; changing his strategy alone cannot create a history in which he actually acquiesces. Hence he also cannot improve.
This direct argument works for both discounted and long-run average payoffs. The outcome gives Ann exactly her minmax payoff and Bob more than his, so it is compatible with the folk theorem for repeated games. A version requiring strict gains above both minmax payoffs is a sufficient condition, and cannot be used to rule out this boundary example.
The definition in this part uses a single Boolean valuation, so the relevant Nash equilibria are pure strategy equilibria of a Boolean game. Use its standard convention that the players' control sets form a set partition of the variables.
Membership follows from an existential choice of a strategy profile and a universal check of all unilateral deviations. Assign payoff one to satisfying a player's goal and zero otherwise. A strategy profile is a Nash equilibrium precisely when, for every player and every alternative Boolean valuation of that player's variables,is true: either the goal is already satisfied or no deviation can satisfy it. Thus the requested property isThe strings encoding , and have polynomial length, and evaluating the bracketed propositional formulas takes polynomial time. Invalid encodings of a player index can simply be ignored by the test. This is the existential second level of the polynomial hierarchy, .
For hardness, reduce the canonical complete problem of deciding a two-block quantified Boolean formulaMake a two-player Boolean game: player 1 controls and has goal ; player 2 controls and has goal . Set the query formula to . The construction has size linear in the input formula.
If an assignment satisfies , combine it with any assignment . Player 1 already satisfies its goal, and player 2 cannot satisfy by any unilateral deviation. Thus is a Nash equilibrium satisfying the query.
Conversely, let be a Nash equilibrium satisfying . Player 2 currently has payoff zero. If some alternative made false, that deviation would satisfy player 2's goal and increase its payoff to one. The Nash equilibrium condition therefore implies . This proves the required equivalence and the polynomial-time reduction.
Together, membership and hardness prove -completeness of existential equilibrium checking in a Boolean game. The reduction works with only two players and one constant goal.
There are unlisted articles, also show them or only show them.