Osmosis is net movement of water across a boundary whose permeability differs for water and relevant solutes. The direction depends on the chemical potential of water, including both dissolved material and pressure. A cell wall can let water reach the cell membrane, yet oppose expansion through turgor pressure. Zero net movement does not mean individual water molecules have stopped crossing.
Imagine pure water on side A and a chemical solution on side B of a semipermeable membrane. At equal temperature and pressure, dissolved particles lower the chemical potential of water in B, and net water transfer initially favors A to B. Retaining the solutes lets water redistribute without simply mixing everything. Increasing B's pressure opposes entry; enough pressure gives thermodynamic equilibrium with unequal solute concentrations. This is why “water moves toward more solute” requires a pressure condition.[ref]
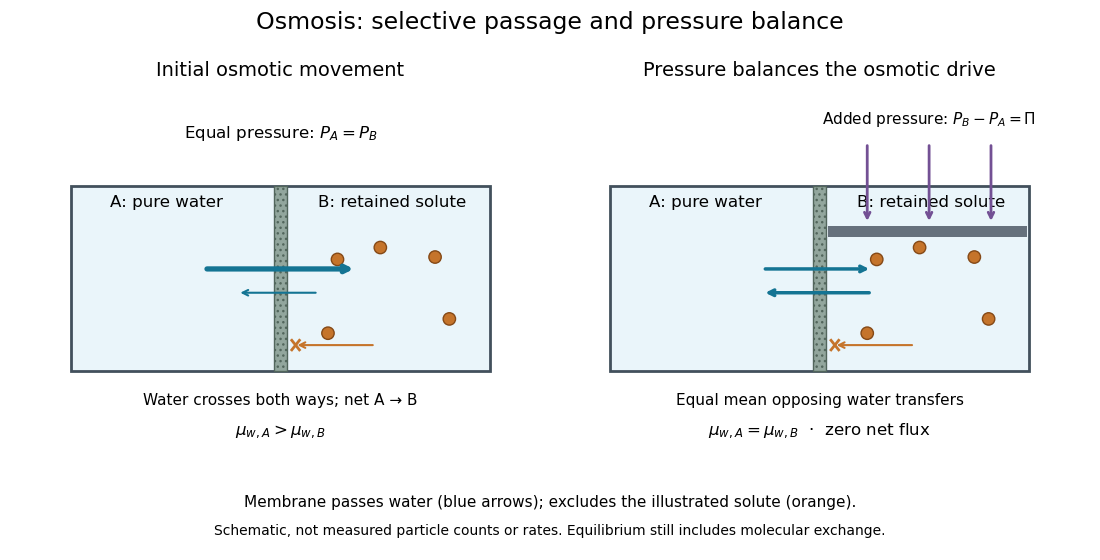

At thermodynamic equilibrium, the chemical potentials of exchangeable water are equal. Individual water molecules still move and cross in both directions, with equal mean opposing transfer rates and zero net flux. A stationary liquid level alone does not prove this: a blocked route can also give no visible transfer. Selective permeability provides a route; water potential supplies the direction, and neither alone determines the speed. The cell wall, turgor pressure and plasmolysis articles show why a living boundary's mechanical support and its selective permeability must be distinguished.
Water potential expresses the chemical potential of water relative to a stated pure-water reference in units of pressure. For a nearly incompressible liquid at fixed temperature, use a constant reference molar volume and writeThe reference is pure water at the same temperature and a chosen pressure . Both sides must use the same reference. Neglecting height differences and interactions with solid surfaces, the approximation isHere is the dimensionless thermodynamic activity of water, the molar gas constant, and the absolute temperature. The natural logarithm is therefore applied to a dimensionless quantity. The pressure contribution increases with pressure; the solute potential is negative when . Across an available passive water route, net water transfer favors higher to lower water potential. The familiar plant description adds effects of height and interactions with solid surfaces when they matter; they are omitted in the two liquid compartments here.[ref]
30.5 Transport of Water and Solutes in Plants. Biology 2e, §30.5, Water Potential, Solute Potential, Pressure Potential and Figure 30.32: component balance and direction of transfer
Adding solute and raising pressure can thus cancel in water potential while each contribution remains nonzero. Equality of water potential does not imply equality of pressure or of every solute concentration. In a supported plant cell, the cell wall permits a positive turgor pressure to balance a negative solute potential; plasmolysis illustrates the opposite loss of support after water leaves.
Solute potential is the contribution to water potential from dissolved material, with pure water assigned zero. In the nearly incompressible description, . In a dilute ideal chemical solution, , where is the osmotic concentration of dissolved particles. Thus solute potential is negative while the corresponding osmotic pressure is positive: . This sign difference distinguishes a contribution to water potential from the compensating mechanical pressure.[ref]
30.5 Transport of Water and Solutes in Plants. Biology 2e, §30.5, Solute Potential: negative concentration contribution
Osmotic pressure is the excess pressure needed on a chemical solution to maintain osmotic thermodynamic equilibrium with pure solvent across a semipermeable membrane. For a nearly incompressible solvent, equality of chemical potential gives . It is an equilibrium property; an observed initial swelling rate is a different measurement.[ref]
osmotic pressure. Gold Book, osmotic pressure: equilibrium definition, solvent activity formula and dilute ideal limit
For a dilute ideal chemical solution of retained particles,Here is the amount of substance of independently dissolved solute particles, measured in moles; is the final volume of chemical solution, not the starting volume of pure solvent. Count the resulting ions separately if a solute dissociates; do not multiply twice if already counts them. With in and in , has units . This resembles the ideal gas law, although the particles here are dissolved in a liquid.
The assumptions are uniform temperature, a dilute ideal chemical solution, a nearly incompressible solvent, and a semipermeable membrane that retains the counted solutes while passing solvent. Association, incomplete dissociation and interactions change the relation between added material and independent particles; nonideal thermodynamic activities invalidate simple particle counting. The formula does not describe a concentrated brine merely because the apparatus contains a membrane.
A short derivation explains why particles are counted. In an ideal mixture, , with the amount of substance of water. If , then and . Substitution gives . This is a dilute-limit approximation, not a claim that water molecules stop moving or that dissolved particles are a gas.
The component of osmotic pressure due to colloidal constituents such as albumin in the circulating fluid.
Measure the pressure difference across a solvent-permeable barrier that retains the solute, at known temperature. For dilute polymers, the zero-concentration intercept of reduced pressure determines the number-average molar mass. Leakage, aggregation and ionic contributions can change the inferred molecular population.
For polymer mass concentration , the leading ideal chain pressure is . Plotting against and extrapolating removes the leading virial correction. The intercept has units of energy per mass; without the measurement temperature it determines , not an absolute molar mass.
Take two reservoirs separated by a semipermeable membrane that passes water and retains one neutral solute. Stipulate , and , equivalent to and . Treat both chemical solutions as dilute and ideal. These are invented model conditions, not measurements or recommended biological conditions.
For pressures measured at the same height beside the membrane, define . The model predictsAt , net water transfer favors A to B. At , the opposing pressure balances the osmotic pressure difference, giving zero net transfer with unequal concentrations. At , the sign reverses and net water transfer favors B to A, toward the more dilute reservoir. Raising pressure changes the total water potential, rather than changing the membrane into a one-way gate.
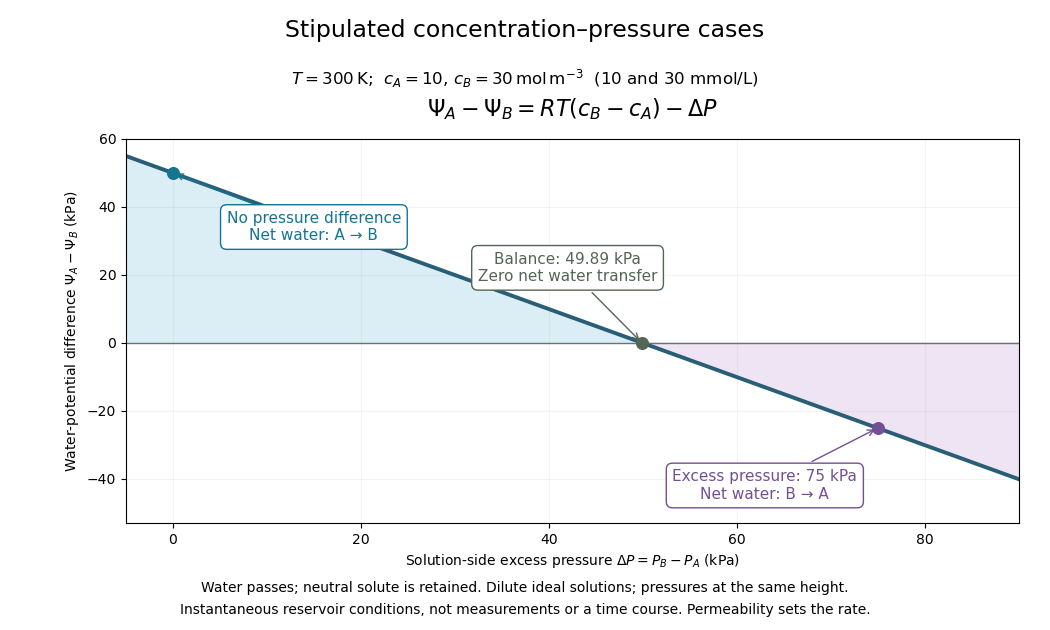

Fixed concentrations require large maintained reservoirs or an instantaneous comparison. In a closed membrane osmometer, entering water causes dilution of the receiving chemical solution and changes its volume; the final balance must use final concentrations. A supported cell wall provides another way to develop the opposing pressure, as explained under turgor pressure.
A membrane osmometer connects osmosis to a visible liquid level or a measured balancing pressure. In a teaching version, a solute-containing pouch is joined to a narrow vertical tube and submerged in external water. Entry increases the enclosed volume and raises the meniscus. Both the column and any stretched pouch can contribute an opposing pressure.
The University of Toronto's Osmosis (Brine) by University of Toronto Department of Physics demonstration (activity Me-012b, Description, steps 1–14) specifies soaking a dialysis membrane tube, tying one end closed and fastening the other around a thistle tube's narrow end. A stand holds the tube. Colored brine is cooled to room temperature and injected using a syringe to reduce bubbles; the pouch is completely immersed in a or beaker of distilled water. A taped marker records the initial level; subsequent meniscus height is the readout. The protocol proposes another pouch containing distilled water as a comparison, and its older instructions explicitly check seals for leaks.[ref]
Osmosis (Brine) by University of Toronto Department of Physics. Osmosis (Brine), Description steps 1–14, water-filled comparison and Old Description A.2: apparatus, readout and leak check
A rise is consistent with net water entry. To infer osmotic pressure quantitatively, use a retained solute and establish a stable equilibrium after accounting for dilution. If both free surfaces are at the same atmospheric pressure, the liquids have approximately equal mass densities , and the pouch adds negligible mechanical load, the hydrostatic pressure difference at membrane height is approximately , where is the meniscus height above the external surface and is gravitational acceleration. This is the liquid-column inference, not a pressure calibration supplied by the Toronto demonstration. For unequal mass densities, compare the two column pressures separately.
Useful additional controls are matched initial levels and geometry, constant temperature, replicate runs, and monitoring external solute to test retention. These are proposed checks, not reported Toronto results. Leaks, trapped bubbles, surface tension in the narrow tube, evaporation and membrane stretching can alter the level. In particular, a dialysis membrane may pass dissolved salt: the brine setup illustrates transient movement but cannot be assumed to retain every dissolved ion. Color improves visibility without proving salt retention. A stationary level can reflect weakening concentration differences or leakage rather than osmotic thermodynamic equilibrium; a rising level alone supplies neither nor a verified value of .
In the dilute ideal particle-count description, osmolarity is the total amount of substance of independently dissolved solute particles per volume of chemical solution: . It includes both membrane-permeating and retained solutes; specifying a particular membrane is unnecessary to count particles. A neutral undissociated solute contributes one particle per molecule, whereas separated ions are counted individually. Common units are or , with one osmole denoting one mole of the counted particles. Osmolality uses mass of solvent instead of volume of chemical solution; the two numerical values should not be identified without the appropriate mass-to-volume conversion.[ref]
Osmosis, Cell Membranes-Structure and Transport, BYU-Idaho. Cell Membranes—Structure and Transport, Osmosis: paragraphs beginning Earlier this semester and Osmolarity is a useful term; total particle counting
This ideal counting definition states its scope: interactions can require a thermodynamic activity description of osmotic pressure. Tonicity asks a different question, namely how that surrounding chemical solution changes a specified biological cell's volume through its particular cell membrane.
Tonicity describes how a surrounding chemical solution changes cellular volume through osmosis. It depends on which solutes remain effectively excluded on the timescale of interest, not simply on the amount of dissolved material. The following comparisons take a functional cell membrane, an initially unpressurized biological cell, and effectively excluded solutes as the reference; rising turgor pressure can oppose entry in a walled biological cell.
Operationally, hypotonic solutions cause sustained swelling, hypertonic solutions sustained shrinking, and isotonic solutions no sustained volume change in the specified passive comparison. State the reference biological cell, membrane properties and observation interval. A permeating solute can transiently change water potential while crossing; after its chemical potential equilibrates, its initial unequal concentrations cannot be treated as a permanently retained osmotic load. Thus equal osmolarities need not imply isotonic solutions. Conversely, a stationary walled biological cell may have unequal osmolarities balanced by turgor pressure.[ref]
Osmosis, Cell Membranes-Structure and Transport, BYU-Idaho. Cell Membranes—Structure and Transport, Osmosis: paragraphs beginning Here is another way and final Note; permeating solutes and transient effects
A permeating solute can cross the specified membrane appreciably during the observation interval. This is a property of a solute-membrane-time comparison, not an immutable label attached to a molecule. Passage can reduce a concentration difference through passive transport while water is also moving; it does not require water to wait.
For an original dilute ideal example, stipulate a flexible model biological cell with retained particles and an external reservoir with retained particles plus freely permeating neutral solute. Initially the total osmolarities are equal. Suppose the permeating solute eventually has equal internal and external concentrations, there is negligible pressure difference, no active transport, and the internal retained particle amount is conserved. The permeating contributions cancel from the final osmotic balance; the internal retained concentration must fall from to . The required volume is twice its initial value. This illustrates an initially equal-osmolarity but hypotonic solution; it assumes the boundary can survive that expansion and predicts no universal time course.
A hypotonic solution favors initial net water entry under the reference conditions above. A susceptible biological cell may undergo osmotic lysis; a sufficiently strong cell wall can instead support turgor pressure.
A hypertonic solution favors initial net water loss under the reference conditions above. In a walled plant cell, enough loss can produce plasmolysis.
An isotonic solution produces no sustained change in cellular volume under the stated comparison conditions. Water can still exchange in both directions.
Osmotic lysis is rupture after excessive water entry and swelling. It is an outcome for susceptible biological cells, not an inevitable response of every biological cell to a hypotonic solution. Cell walls can bear the resulting load, and cellular mechanisms can regulate water balance. A protoplast challenge tests a particular preparation under particular conditions.
Articles by others on the same topic
There are currently no matching articles.