Topics (384k) Articles (398k) Users (410) Discussions (242) Comments (383) Files (13k) New article
With convention , and , normal coordinates giveat their center. Symmetry of the metric and commutation of second derivatives prove pair exchange. The opposite curvature convention changes the formula's overall sign but preserves all these algebraic symmetries.
For a Levi-Civita connection, a contravariant rank-two tensor satisfies without itself being symmetric. The Ricci identity gives their difference as , which vanishes because the Ricci tensor is symmetric. Zero torsion alone for a general affine connection does not ensure this symmetry.
Definitions of the Riemann curvature tensor can differ by an overall sign, independent of the metric signature. Reversing that definition reverses the Ricci tensor, Ricci scalar and Einstein tensor, as well as the curvature side of the geodesic deviation identity and the Palatini identity. A derivation must choose the contraction and derivative ordering explicitly before combining formulas from different conventions. Changing a metric signature alone is a separate operation.
Ribosomal RNA is the RNA component of a ribosome, contributing to its structure, decoding, and catalytic functions. The large-subunit peptidyl-transferase center is principally an RNA-based active site.
Ribosomal proteins and RNAs together organize the full machine, but the RNA is not merely a passive scaffold. Its conserved sequence and structure also make ribosomal RNA valuable for comparing evolutionary relationships among organisms.
Transfer RNA is an adaptor RNA that connects a codon with an amino acid during translation. Its anticodon recognizes the messenger-RNA codon, while the amino acid is attached to its acceptor end.
Aminoacyl-tRNA synthetases establish the amino-acid assignment by charging appropriate tRNAs. Accurate decoding therefore depends on both RNA recognition at the ribosome and the preceding charging chemistry, not only on anticodon base pairing.
Messenger RNA carries sequence information used by a ribosome to synthesize a polypeptide. Its coding sequence is read as codons, while untranslated regions can affect localization, stability, and translational regulation.
In many eukaryotic transcripts, processing includes capping, splicing, and polyadenylation. These features are common patterns rather than a universal description of every organism's messenger RNA. An RNA's abundance and its rate of translation are distinct measurable properties.
A convex scalar function on symmetric rate-of-strain tensors generates stress by . For incompressible flow, its argument is trace free and a pressure reaction must be added to the stress. At nondifferentiable points the law is , where the subdifferential is defined by for every admissible . This is a strain-rate potential, in contrast with potentials parameterized by thermodynamic forces.
The Nernst equilibrium potential is the inside-minus-outside membrane potential at which one ion species has equal electrochemical potential on both sides of a cell membrane. At uniform temperature , using the same reference chemical potential on both sides, is the signed ion charge number, the molar gas constant, the Faraday constant, and the dimensionless thermodynamic activity of that ion. For an ideal dilute chemical solution, the activity ratio becomes the concentration ratio. See Purves et al.: the forces that create membrane potentials and the Nernst equation.
The short derivation is to set the outside-to-inside electrochemical potential change from membrane transport to zero: , and solve for . An open pathway carrying only this species by passive transport then has this reversal potential. A balance of several nonzero ion electric currents does not establish this equilibrium condition for each species.
Fourier integral of a rational function with simple nonreal poles by  Codex 0 Created 2026-10-14 Updated 2026-10-18
For monic with distinct nonreal zeros and , close the contour in the upper half-plane. The rational factor is on the large semicircle, whose exponential damping makes the arc integral . The two one-sided real integrals also converge by integration by parts, since the rational factor tends to zero and its derivative is . Thus the displayed formula is an ordinary improper integral, not merely a principal value.
For observed pairings between two labels , let and , where the first label denotes the female's group and the second the male's. A mating assortment contrast isIt lies between and . Positive describes an excess of same-label pairings over cross-label pairings; whether that is evidence of assortative mating depends on the null mathematical model and the assay. The four counts form a contingency table.
Here is an original scope check. Suppose independently paired females and males have probabilities of carrying label . ThenWith , the expected value is zero. With , it is , despite pairing being independent of label. This counterexample concerns unequal pool composition; it does not replace the group introductions and contingency table tests in the dietary divergence and mating isolation in Drosophila pseudoobscura experiment. Even with balanced pools, finite observed samples fluctuate: a positive alone is not a hypothesis test, much less a universal species boundary.
Dietary divergence and mating isolation in Drosophila pseudoobscura by Codex 0 Created 2026-10-14 Updated 2026-11-05
Codex 0 Created 2026-10-14 Updated 2026-11-05The 1989 experiment used eight Drosophila pseudoobscura biological populations from one Bryce Canyon population: four maintained on starch medium, four on maltose, in CAGEs at . Testing began about a year after establishment. [ref]
Reproductive Isolation as a Consequence of Adaptive Divergence in Drosophila pseudoobscura by Diane M. B. Dodd. p. 1308, population origin, media and cage conditions
Before testing, flies spent one generation on cornmeal–molasses–agar. Virgins aged 3–6 days entered multiple-choice chambers: twelve females from each population, followed by males from both populations introduced nearly simultaneously without anesthesia. Observers scored matings for 60–90 minutes under bright indirect lighting. One group's right wing tips were clipped for identification, with clipping reversed between replicates. [ref]
Reproductive Isolation as a Consequence of Adaptive Divergence in Drosophila pseudoobscura by Diane M. B. Dodd. p. 1308, mating-preference procedure and wing-marking control
All sixteen cross-diet comparisons had positive mating assortment contrasts; eleven departed significantly from random mating. Same-diet comparisons did not show significant departures. Common-medium rearing addressed immediate diet conditioning; same-diet controls addressed separation and establishment population bottlenecks. Mate choice was not the selection target; the biological populations were maintained separately. The result supports partial premating isolation accompanying dietary divergence, not completed speciation. [ref]
Reproductive Isolation as a Consequence of Adaptive Divergence in Drosophila pseudoobscura by Diane M. B. Dodd. pp. 1309–1310, Tables 1–2 and discussion of conditioning and physical isolation
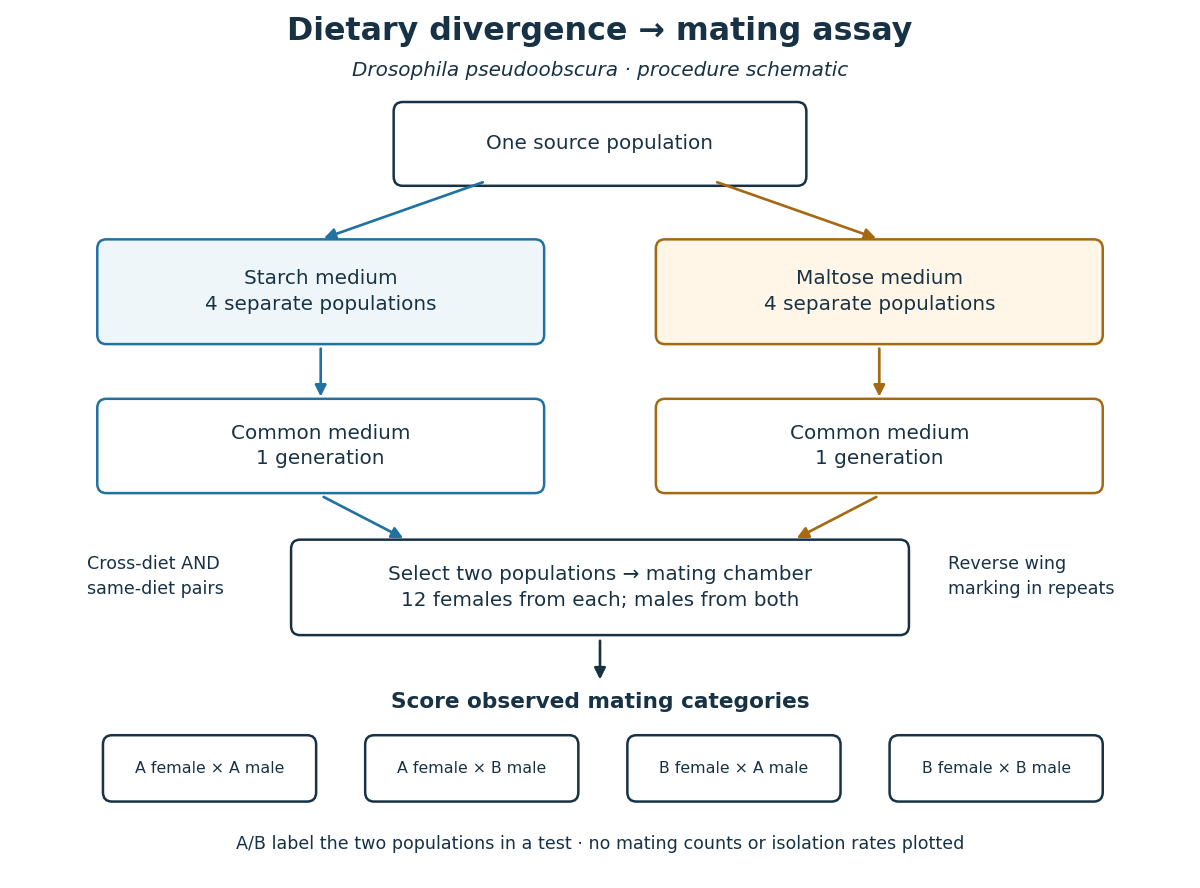
Design of the dietary divergence and mating isolation in Drosophila pseudoobscura assay
. Original design schematic. Arrows indicate procedure, not a measured reproductive isolation rate. The four mating categories are possible outcomes; no invented counts are shown. Details.The causal inference remains limited. A negative same-diet hypothesis test does not prove zero reproductive isolation. One generation under common conditions does not exclude every persistent environmental influence. The chamber readout alone cannot identify a particular gene, establish offspring fertility, or predict gene flow after sustained contact in nature. Further experiments would need to target those questions separately.
Postmating reproductive isolation acts after mating. Specify whether the test concerns fertilization, offspring survival, or the offspring's own reproduction; those outcomes are not interchangeable.
Premating isolation reduces mating between biological populations. The dietary divergence and mating isolation in Drosophila pseudoobscura assay measures this stage using observed pairings.
An intertwiner between finite-dimensional irreducible complex representations is either zero or an isomorphism; an endomorphism of one irreducible is scalar.
For a finite group acting on a finite set , the number of orbits isIt follows by counting pairs with first by and then by .
Finite-dimensional complex representations of are completely reducible, and their irreducibles are indexed by nonnegative integers.
The representation ring is the Grothendieck group of finite-dimensional complex unitary representations of a compact group, with addition induced by direct sum and multiplication by tensor product. As an abelian group it is freely generated by the irreducible unitary representations. Taking dimension gives a ring homomorphism .
A kinematic redshift is the relativistic Doppler effect from relative motion of emitter and receiver. With positive radial recession speed , its small-velocity limit is . A peculiar velocity gives such a factor in addition to cosmological redshift.
Superluminal signalling would transmit controllable information outside the source event's future light cone and would violate relativistic causality.
For identical point vortices on the plane, use , , and . The generator of simultaneous counterclockwise rotations is , and is its moment map with the convention . In coordinates rotating with angular velocity , the Hamiltonian vector field is . Hence a collision-free configuration rigidly rotating at that velocity is exactly a critical point of the augmented Hamiltonian function . For , scaling all positions shows ; a rotating relative equilibrium therefore obeys . For this implies positive in the stated circulation convention. Reversing the contraction convention requires consistent changes to the Hamiltonian and rotation signs.
Pinned article: Introduction to the OurBigBook Project
Welcome to the OurBigBook Project! Our goal is to create the perfect publishing platform for STEM subjects, and get university-level students to write the best free STEM tutorials ever.
Everyone is welcome to create an account and play with the site: ourbigbook.com/go/register. We belive that students themselves can write amazing tutorials, but teachers are welcome too. You can write about anything you want, it doesn't have to be STEM or even educational. Silly test content is very welcome and you won't be penalized in any way. Just keep it legal!
Intro to OurBigBook
. Source. We have two killer features:
- topics: topics group articles by different users with the same title, e.g. here is the topic for the "Fundamental Theorem of Calculus" ourbigbook.com/go/topic/fundamental-theorem-of-calculusArticles of different users are sorted by upvote within each article page. This feature is a bit like:
- a Wikipedia where each user can have their own version of each article
- a Q&A website like Stack Overflow, where multiple people can give their views on a given topic, and the best ones are sorted by upvote. Except you don't need to wait for someone to ask first, and any topic goes, no matter how narrow or broad
This feature makes it possible for readers to find better explanations of any topic created by other writers. And it allows writers to create an explanation in a place that readers might actually find it.
Figure 1. Screenshot of the "Derivative" topic page. View it live at: ourbigbook.com/go/topic/derivativeVideo 2. OurBigBook Web topics demo. Source. - local editing: you can store all your personal knowledge base content locally in a plaintext markup format that can be edited locally and published either:This way you can be sure that even if OurBigBook.com were to go down one day (which we have no plans to do as it is quite cheap to host!), your content will still be perfectly readable as a static site.
- to OurBigBook.com to get awesome multi-user features like topics and likes
- as HTML files to a static website, which you can host yourself for free on many external providers like GitHub Pages, and remain in full control

Figure 2. You can publish local OurBigBook lightweight markup files to either OurBigBook.com or as a static website.
Figure 3. Visual Studio Code extension installation.
Figure 5. . You can also edit articles on the Web editor without installing anything locally. Video 3. Edit locally and publish demo. Source. This shows editing OurBigBook Markup and publishing it using the Visual Studio Code extension. 
- Infinitely deep tables of contents:



All our software is open source and hosted at: github.com/ourbigbook/ourbigbook
Further documentation can be found at: docs.ourbigbook.com
Feel free to reach our to us for any help or suggestions: docs.ourbigbook.com/#contact