Past exam of the zoology course of the University of Cambridge 2025 Paper zl3 2 Solution by  Codex 0 2026-10-20
Both conflicts arise because family members value the same resource differently, but they concern different decisions. Sibling rivalry concerns allocation among offspring, whereas parent-offspring conflict concerns a parent's allocation relative to what an offspring would favour. Their consequences interact: offspring compete with one another inside a parental provisioning system that their own demands can also alter.
The basic mechanism is unequal genetic relatedness to the beneficiaries of an action. An offspring values its own additional survival or reproduction more strongly than an equal gain to a sibling. A parent, under a simple symmetric pedigree, is equally related to each of its offspring and can favour an allocation that maximizes their combined contribution. Neither statement implies that an offspring should demand everything: diverting resources from relatives can reduce its inclusive fitness. These differing interests underlie the original theory of parent-offspring conflict.[ref]
Parent-Offspring Conflict by Robert L. Trivers. 1974, theory of investment, sibling costs and the duration of care
Consider an explicit illustrative model. Let investment produce a direct offspring benefit and an opportunity cost measured in lost equivalent fitness contributions of other offspring. Assume a single parent, equal value of current and future offspring, no inbreeding, and relatedness between the focal offspring and those losing resources. After dropping a common parental relatedness factor, the parent's objective is , whereas the offspring's is . Interior optima therefore satisfyWith diminishing marginal benefits and , the offspring typically favours more investment. In particular, the range contains increments favoured by the offspring but opposed by the parent. For full siblings under the stated pedigree, ; for maternal half-siblings, . These values are not universal constants for all family structures, and parent survival, reproductive value and density dependence can alter the effective costs.
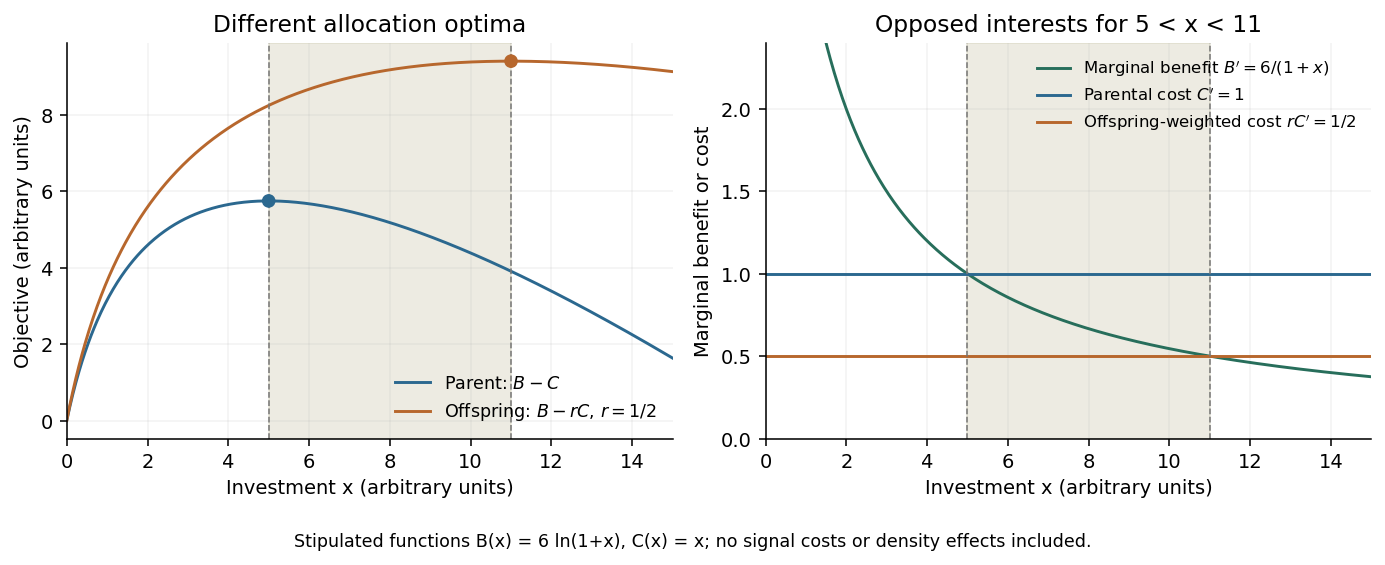
An original illustrative allocation model separates parental and offspring optima
. Chosen functions and give a parental optimum at and a full-sibling-weighted offspring optimum at . The shaded interval contains increments whose marginal benefit is below the parental opportunity cost but above the offspring-weighted cost. These are stipulated functions and arbitrary units, not empirical measurements. Details.
Sibling rivalry selects on relative access; parent-offspring conflict can also change the total supply. If one nestling obtains a larger fraction of a fixed food delivery, its sibling loses directly. Selection can favour size advantages, advantageous positions, earlier hatching or more effective solicitation. Severe asymmetries can permit siblicide or brood reduction. By contrast, a stronger demand directed at a parent can increase food delivery to the brood, potentially benefiting siblings too. The same begging behaviour can therefore redistribute a fixed supply and alter parental effort, with different consequences in each case.
A parent's preferred distribution need not be equal. A marginal food item may produce more surviving descendants when given to a smaller hungry chick, or to a larger chick that alone can survive a severe shortage. Parental allocation can consequently mitigate sibling asymmetry in one environment and reinforce it in another. Asynchronous hatching and brood-size adjustment are plausible parental means of structuring that contest; whether a particular asymmetry is an adaptation, a constraint or an offspring-driven outcome needs evidence. A parent's tolerance of brood reduction is not proof that every aggressive act serves parental interests.
Over evolutionary time, sibling rivalry can affect competitive morphology, growth schedules, solicitation, nest position and the survival distribution within broods. Parent-offspring conflict can affect the amount and duration of care, offspring demand, parental responsiveness, weaning schedules and the trade-off between current and future reproduction. Neither conflict predicts unlimited escalation. Energetic expenditure, injury, predation risk and losses to relatives can make competitive effort costly even when it obtains a larger resource share.
Information can produce compromise as well as waste. An offspring usually has private information about its hunger, while the parent integrates brood condition with its own prospects. In a costly-signalling model, offspring in greater need gain more from additional resources, so differing incentives can support informative solicitation at equilibrium. Such a result is conditional on the cost and benefit functions; it does not mean all begging is perfectly honest or that energetic expenditure alone establishes honesty.[ref]
Signalling of need by offspring to their parents by H. C. J. Godfray. 1991, primary signalling model and its assumptions
Signals can also be aimed at siblings. Experiments on barn owls found that nestlings reduced vocalization when a rival was hungrier, increased it after that rival was fed, and altered calling with experimental brood size. These calls occurred when parents were absent. They support sibling negotiation: assessing relative willingness to contest a future prey item can avert some unnecessary escalation. The experiment therefore cautions against treating every nestling call as a demand directed at the parent.[ref]
Barn owl (Tyto alba) siblings vocally negotiate resources by Alexandre Roulin and others. 2000, hunger and brood-size manipulations
A further consequence is coevolution among parental and offspring response rules. A demand phenotype expressed in young becomes part of the selective environment of provisioning adults, while parental allocation changes the returns to offspring competition. The same individual can experience both roles at different life stages, and genetic correlations between demand and care can constrain independent optimization. Thus observed care can be a compromise maintained by interacting strategies rather than the optimum of either party in isolation.
The comparison is consequently about overlapping arenas of selection. Sibling rivalry chiefly determines who obtains care, while parent-offspring conflict also determines how much care is supplied and when it ends. Both can generate competitive adaptations and costs, but both can also generate assessment, contingent responses and restraint. A strong empirical test must separate changes in total provisioning from redistribution, measure lifetime consequences rather than only immediate feeding success, and manipulate relatedness or information without simultaneously changing need.
Past exam of the zoology course of the University of Cambridge 2025 Paper zl3 1 Solution by Codex 0 2026-10-20
Codex 0 2026-10-20The strength of conflicting interests, opportunities for exploitation and receiver defences matter more than the species boundary itself. Many striking examples occur between species, where shared descent usually supplies little inclusive fitness restraint. However, competition for mates and resources also creates substantial conflict within a species, including between relatives. The available examples do not establish a universal numerical ranking of the two settings.
A useful distinction is between deceptive signalling and the broader category of behavioural manipulation. A deceptive display exploits a receiver response in a context in which that response no longer provides the normally associated benefit. Manipulation also includes changing another organism's physiology or behaviour without conveying misleading information. Neither definition requires conscious lying or knowledge of another individual's beliefs. Ordinary persuasion is not a helpful biological criterion: the relevant comparison is between the reproductive success consequences for sender and receiver, relative to appropriate alternatives.
Between species, exploitation can borrow a response that is maintained for another reason. A predator can mimic an attractive prey cue; a parasite can exploit a host's provisioning or avoidance mechanism; and a plant can attract a pollinator without providing the expected reward. Such interactions can favour sensory exploitation and aggressive mimicry. Receiver resistance is selected when the losses outweigh its costs, but resistance need not eliminate deception. Rejecting a genuine mate or ignoring a real predator can be more costly than occasionally accepting a false signal.
In fork-tailed drongos, observations and playback experiments showed that false alarm calls can make other foragers abandon food, which the drongo steals. Receivers habituated to repeated alarms, while switching among alarm types, including mimicked calls, helped sustain responses. This demonstrates both an exploiter benefit and a receiver counterresponse. It does not require an inference that drongos attribute beliefs to their victims.[ref]
Deception by Flexible Alarm Mimicry in an African Bird by Tom P. Flower and others. 2014, field observations and playback tests of alarm variation and habituation
A different mechanism occurs in the orchid Ophrys sphegodes. Chemical analyses and behavioural tests implicated a floral blend matching components of female Andrena nigroaenea sex pheromone in attracting males that transfer pollen during attempted mating. Here deception exploits a reproductive response maintained in the pollinator's own species, rather than a communication system jointly serving orchid and bee. The orchid example demonstrates a specific mechanism, not the frequency of deception across all pollination systems.[ref]
Orchid pollination by sexual swindle by Florian P. Schiestl and others. 1999, floral chemistry and field behavioural tests
Behavioural manipulation can go beyond signals. In experimental comparisons, Toxoplasma gondii-infected rats showed altered responses to cat-associated odours, sometimes approaching locations avoided by uninfected rats. This is consistent with a transmission-enhancing effect because felids are the parasite's definitive hosts. However, an odour preference assay does not itself demonstrate increased predation by cats, greater parasite transmission, or that every infection-associated behavioural change is an adaptation. Illness, host defence and collateral pathology remain alternative explanations requiring separate tests.[ref]
Fatal attraction in rats infected with Toxoplasma gondii by M. Berdoy and others. 2000, experimental odour responses and interpretation
Within species, common ancestry does not imply identical interests. A mating partner may benefit from extra copulations that impose costs on the other partner; competitors may benefit by concealing food or exaggerating fighting ability; offspring may demand more care than maximizes parental lifetime reproductive success. Kin selection weakens some conflicts because harming a relative can also reduce an actor's inclusive fitness, but it does not generally remove them. For an unrelated rival, even that indirect cost may be absent.
Male topi provide a direct counterexample to the claim that deceptive communication is mainly possible across species. Field observations and playback work associated false alarm snorts with retaining receptive females within male territories and obtaining mating opportunities. Alarm responsiveness remains useful to females when a predator really is present, allowing a sexual conflict to exploit an otherwise protective response. The relevant opposition is male versus female mating interests, despite their membership of the same species.[ref]
Male Topi Antelopes Alarm Snort Deceptively to Retain Females for Mating by Jakob Bro-Jørgensen and Wiline M. Pangle. 2010, alarm context, female responses and mating consequences
There are also reasons why repeated interactions can restrain exploitation in either setting. A receiver can learn, recognize individuals, stop responding, abandon a partner, or impose a cost on it. In many mutualisms, both parties gain from preserving the association, even though each would benefit from obtaining more while supplying less. Conversely, within-species relatedness need not be high, and a short-lived encounter may give little opportunity for retaliation. Thus “between species” is an imperfect proxy for the underlying distribution of benefits, costs, encounter rates and alternatives.
To establish comparative prevalence, one would need a denominator: deceptive acts per interaction, the fraction of signal types exploited, the proportion of individuals using manipulation, or the number of independent evolutionary origins. Those measures can rank systems differently. Sampling would also need to control for observation effort, interaction frequency, detection probability and phylogenetic nonindependence. A concealed false signal can be harder to identify than an obvious parasite-induced change; spectacular cases attract disproportionate study.
The defensible prediction is conditional. Exploitation should be favoured where it increases the actor's reproductive success, the receiver's defences are ineffective or costly, and countervailing relatedness or future-interaction costs are small. Interspecific antagonism often meets these conditions, but so do some intraspecific sexual and competitive interactions. A comparative answer should therefore explain those conditions and acknowledge that the examples alone cannot settle a universal prevalence claim.
Past exam of the zoology course of the University of Cambridge 2025 Paper zl1 6 Solution by Codex 0 2026-10-20
Codex 0 2026-10-20The Holocene history combines natural climatic and geographic filtering with increasingly strong human restructuring through hunting, habitat change, domestication, introductions and conservation. The balance varies through time and between Britain and Ireland. The Holocene begins approximately 11.7 thousand calibrated years before present; for radiocarbon dating, “present” conventionally means 1950. Uncalibrated radiocarbon ages must not be silently treated as calendar ages.
At the beginning, warming following the last glaciation changed vegetation and the distribution of food and cover. Open, cold-adapted assemblages gave way to a changing mixture of woodland, wetland and open-habitat mammals. Rising seas progressively restricted natural colonization; Britain retained connections to continental Europe later than Ireland's faunal assembly can simply be assumed to have done. The modern Irish fauna is therefore not a complete British fauna subsequently pruned by identical extinctions. A missing Irish species may never have colonized, rather than having been exterminated there. pollen analysis, stratigraphy and directly dated bones help distinguish habitat change from collecting gaps.
Chronology prevents an equally misleading division into wholly “Pleistocene” losses and wholly modern survivors. Some conspicuous cold-stage mammals, such as the woolly rhinoceros, disappeared from Britain before the Holocene and should not automatically be included in a Holocene hunting-extinction list. Conversely, directly dated giant deer from the northern Irish Sea basin demonstrate early Holocene survival of a lineage once thought to have disappeared regionally earlier. [ref]
Survival of the Irish elk into the Holocene by Silvia Gonzalez and others. Nature 405, pp. 753–754; directly dated giant deer from the northern Irish Sea basin
A date from one part of this region does not establish persistence everywhere in Ireland or Britain. Local disappearance, regional disappearance and global extinction are different endpoints; environmental deterioration and human activity need to be evaluated at the appropriate geographic and chronological scale.Later prehistory saw a profound change in mammalian abundance as farming spread. Domestic cattle, sheep, goats and pigs became major components of archaeological assemblages and living biomass. Grazing, clearance and woodland management altered habitat for wild herbivores and their predators; settlement and stored food also favoured commensal rodents. This was more than adding several species to an unchanged ecosystem. Distinguishing domestic from wild forms requires skeletal comparisons, context and, where available, Ancient DNA and stable isotope analysis. A large number of livestock bones in a settlement midden is evidence of human use, not a direct census of every mammal in the surrounding landscape.
Losses of large native species were staggered. British aurochs, wild boar, lynx, brown bears, beavers and wolves disappeared at different times through combinations of hunting, persecution, habitat transformation and habitat fragmentation. The list cannot be transferred intact to Ireland: a secure native record must be established for each taxon, and a late imported specimen does not demonstrate an earlier indigenous population. Small and elusive species are also less visible in many archaeological deposits, so the absence of their remains should not be equated with a known extinction date.
The dated British lynx record is especially instructive. Survival into the early medieval period makes an explanation based solely on warming at the start of the Holocene inadequate. Human habitat change and direct or indirect persecution become more plausible proximate causes, although the last dated specimen cannot identify which pressure killed the final population. [ref]
New evidence for the occurrence of Eurasian lynx (Lynx lynx) in medieval Britain by David A. Hetherington and others. Journal of Quaternary Science 21, pp. 3–8; directly dated lynx bone and implications for extinction causes
brown bear history is less tidy: review of the British evidence supports either late Neolithic/early Bronze Age or early medieval extinction, and later archaeological bear remains can represent imported captive animals rather than surviving wild populations. [ref]The presence of the brown bear Ursus arctos in Holocene Britain: a review of the evidence by Hannah J. O'Regan. assessment of native survival versus imported animals and alternative extinction chronologies
Traditional stories of the “last wolf” likewise require caution; historically documented persecution is much stronger evidence of human pressure than an unverified exact last-kill year.Human transport makes apparent continuity equally uncertain. Combined skeletal, Ancient DNA and phylogeography evidence indicates a complex Irish red deer history involving prehistoric and recent introductions, rather than simple uninterrupted survival of every modern population from the last glaciation. Neolithic-era records and the contrast between older Kerry-associated ancestry and many recent stocks must be interpreted with sampling gaps in mind. [ref]
Phylogeographic, ancient DNA, fossil and morphometric analyses reveal ancient and modern introductions of a large mammal: the complex case of red deer (Cervus elaphus) in Ireland by Ruth F. Carden and others. Quaternary Science Reviews 42, pp. 74–84; Neolithic record, ancient DNA and recent introductions
Modern distribution alone cannot distinguish an ancient native population, an early species translocation, and a recent estate introduction. Each may require a different conservation interpretation even if all animals bear the same species name.fallow deer provide a clearer example of deliberate species translocation. Integrated archaeological and biomolecular research traces Roman movements and later medieval redistribution, including the British history of introduction and reintroduction. [ref]
The 10,000-year biocultural history of fallow deer and its implications for conservation policy by Karis H. Baker and others. British Roman introductions and medieval translocations; combined biomolecular and archaeological evidence
Managed rabbits and later introductions of sika deer, muntjac, grey squirrels and American mink further altered assemblages. Some escaped from breeding or management; others were deliberately released. Historical records establish routes and timing that cannot be deduced from climatic suitability alone. Modern invasions are thus a continuation of human-mediated assembly, with potentially stronger effects because transport crosses barriers that once limited colonization.The replacement of red squirrels by grey squirrels illustrates multiple interacting mechanisms. interspecific competition for resources can matter, but experimental infection demonstrated severe infectious disease in red squirrels with little detectable effect on grey squirrels, supporting a role for squirrelpox in some declines. [ref]
Parapoxvirus causes a deleterious disease in red squirrels associated with UK population declines by Daniel M. Tompkins and others. Proceedings of the Royal Society B 269, pp. 529–533; contrasting experimental susceptibility of red and grey squirrels
That experiment establishes differential susceptibility; it does not show that every field decline is caused by the virus. A field test must establish infection exposure as well as squirrel abundance and account for habitat and competitor density. Likewise, recovery of pine martens in Ireland has been associated with declines of grey squirrels and recovery opportunities for red squirrels; the evidence is informative but a spatial association alone is not a controlled demonstration that predation explains every local change. [ref]Population crash in an invasive species following the recovery of a native predator: the case of the American grey squirrel and the European pine marten in Ireland by Emma Sheehy and others. Biodiversity and Conservation 23, pp. 753–774; distributional changes associated with pine marten recovery
Recent protection, woodland recovery and reintroductions also allow people to reverse some earlier losses. Such recoveries do not recreate a unique pristine baseline: a “native” reference chosen at the beginning of the Holocene, before farming, or before modern introductions gives different assemblages. The same applies to interpreting recovering coastal populations; marine and terrestrial records need their own detection and exploitation histories. Reliable attribution combines directly dated remains, habitat evidence, historical documentation and demographic or experimental tests, with explicit allowance for preservation and survey effort.
Climate and access strongly shaped early Holocene assembly; later changes increasingly reflect farming, persecution and transport, with modern infectious disease and conservation adding further layers. Human influence is therefore pervasive, but neither every absence nor every change in abundance can be assigned to humanity without establishing when and where the change occurred.
Past exam of the zoology course of the University of Cambridge 2025 Paper zl1 5 Solution by Codex 0 2026-10-20
Codex 0 2026-10-20Living great apes are indispensable comparative evidence, but none is a preserved version of the Pan–Homo last common ancestor. The ancestor was a population with its own combination of traits, and every living descendant has subsequently evolved. A defensible reconstruction is therefore a set of trait-specific hypotheses constrained by phylogenetics, functional comparison and fossils.
The comparison starts with relationships. Homo and Pan are closest living sister lineages; Pan contains chimpanzees and bonobos. Gorilla provides a more distant comparison, and Pongo a more distant one again. Humans are themselves great apes, rather than a group standing outside them. A character shared by Pan and Homo may have been inherited from their last common ancestor, but it can also have changed in either lineage or arisen in parallel. A shared feature of Pan and Gorilla does not automatically reconstruct the ancestor either: it may be ancestral, convergent, or retained in some branches and lost in others.
Living great apes are especially valuable because their soft tissues, growth, behaviour and mechanical performance can be studied. Muscle paths, joint motion and hand loading can make competing functional interpretations of a fossil wrist testable. Observing climbing and terrestrial movement establishes which combinations are mechanically possible; it also exposes the inadequacy of labelling a whole animal simply “arboreal” or “terrestrial”. Appropriate controls compare individuals of different ages and sexes, adjust for body size, record substrate and loading, and distinguish performance in captivity from behaviour in the wild. A surface that resembles another surface is weak functional evidence unless its position in the complete joint and the range of loads are considered.
The same accessibility creates temptations. chimpanzee locomotion, male coalitions or territorial behaviour cannot be transferred wholesale to the common ancestor. bonobos demonstrate variation within Pan, not a second unchanged ancestral template. Ecology, group composition, developmental plasticity and histories of selection differ among living populations. Current behaviour can generate hypotheses about feasible ancestral social systems, but proving that a particular ancestral behaviour existed requires additional evidence; most social behaviours do not fossilize. Treating the contrast as a choice between a uniformly aggressive chimpanzee ancestor and a uniformly peaceful bonobo ancestor replaces biology with caricature.
knuckle-walking illustrates the genuine scientific alternatives. One reconstruction takes the shared use of knuckle support in Pan and Gorilla as evidence for an ancestral condition, with later loss or modification in the hominin lineage. wrist features in early hominins have been interpreted as retained support for that hypothesis. [ref]
Evidence that humans evolved from a knuckle-walking ancestor by Brian G. Richmond and others. Nature 404, pp. 382–385; wrist characters interpreted as retained knuckle-walking adaptations
A competing study emphasized differences in the development and functional organization of chimpanzee and Gorilla wrists, consistent with independent origins of their knuckle-walking systems. [ref]Independent evolution of knuckle-walking in African apes shows that humans did not evolve from a knuckle-walking ancestor by Tracy L. Kivell and others. PNAS 106, pp. 14241–14246; contrasts between chimpanzee and gorilla wrist development and function
Similar external posture can therefore conceal distinct load-bearing arrangements. Neither simply counting two living knuckle-walking genera nor quoting the conclusion of one comparative study settles the ancestral condition. The inference depends on biological homology, functional interpretation and inclusion of relevant extinct forms.Ardipithecus ramidus, approximately 4.4 Ma, is particularly important because its skeleton combines a grasping great toe and arboreal capabilities with anatomy interpreted as supporting terrestrial bipedalism. The authors argued that its hands and feet did not represent an unchanged modern chimpanzee locomotor package. [ref]
Ardipithecus ramidus and the paleobiology of early hominids by Tim D. White and others. Science 326, pp. 75–86; 4.4 Ma skeleton and locomotor mosaic
This weakens a reconstruction that derives early hominins by merely standing a modern chimpanzee upright. However, Ardipithecus lived after the inferred Pan–Homo divergence; its features may include specializations of its own. Its proposed hominin position and functional reconstruction must also be evaluated against incomplete preservation and distortion, especially in the pelvis. It is evidence about a nearby branch, not direct observation of the common ancestor.Older Miocene apes extend the comparison beyond surviving lineages. Pierolapithecus, approximately 12.5–13 Ma, combines an upright-trunk construction (orthogrady) with hand anatomy lacking the complete suspensory specialization of some living apes. [ref]
Pierolapithecus catalaunicus, a new Middle Miocene great ape from Spain by Salvador Moyà-Solà and others. Science 306, pp. 1339–1344; orthograde trunk and contrasting hand morphology
The example shows that trunk posture, climbing and suspensory locomotion can evolve as a mosaic. Its exact position is debated, and it is not thereby identified as the Pan–Homo ancestor. Rather, extinct combinations expand the set of plausible ancestral forms and can reveal that a feature widespread among living apes was assembled in stages.Genetic evidence establishes relationships and helps constrain timing, but a molecular divergence estimate is not a fossil anatomical reconstruction. Estimates are sensitive to mutation rate, calibration and generation interval. Pedigree observations of wild chimpanzees and Gorilla demonstrate why substituting one universal generation length can shift the inferred dates of great-ape divergences. [ref]
Generation times in wild chimpanzees and gorillas suggest earlier divergence times in great ape and human evolution by Kevin E. Langergraber and others. PNAS 109, pp. 15716–15721; pedigrees, generation intervals and divergence-time sensitivity
A gene tree can also coalesce before a population split, and incomplete lineage sorting means that not every genomic region follows the species branching order. There is consequently no reason to force every candidate fossil into an overly precise split date selected from one molecular estimate.The best procedure is to specify competing ancestral states and their predictions: for example, whether a particular wrist character should accompany habitual knuckle support, or whether an inferred climbing apparatus requires suspensory finger proportions. Score those characters across Pan, Homo, Gorilla, Pongo and well-preserved fossil taxa; examine sensitivity to uncertain character coding and alternative fossil placements. Related features must not be counted as a large number of independent confirmations when they are mechanically or developmentally coupled. Extant-only ancestral state reconstruction is especially vulnerable to the extinction of lineages that possessed combinations absent today.
Living great apes supply the comparative mechanics, development and diversity needed to interpret fossils; fossils prevent the living sample from dictating a false ancestral stereotype. A cautious composite reconstruction, with separate uncertainty for posture, hand use, diet and behaviour, is more defensible than choosing one living species as the ancestor's complete anatomical and social model.
Past exam of the zoology course of the University of Cambridge 2025 Paper zl1 4 Solution by Codex 0 2026-10-20
Codex 0 2026-10-20Repeated movements out of Africa are compatible with a predominant shared source for the ancestry of living non-Africans. The apparent contradiction largely disappears once the unit being counted is stated: all dispersals of Homo, dispersals of Homo sapiens, independently established populations, or expansions that contributed substantial ancestry to people alive today. These are different historical claims.
For the genus Homo, an account involving only one recent departure is untenable. Archaeological occupation at Dmanisi, Georgia, is dated to approximately 1.85–1.78 Ma, long before the late Pleistocene expansion of Homo sapiens. The earliest occupation levels must be distinguished from the somewhat younger hominin-bearing deposits: the site is not a single instantaneous event. Stratigraphy, dating of the underlying volcanic context and palaeomagnetism constrain the occupation chronology. [ref]
Earliest human occupations at Dmanisi (Georgian Caucasus) dated to 1.85–1.78 Ma by Reid Ferring and others. Results, stratigraphy and palaeomagnetic chronology; distinguish earliest occupation from hominin-bearing beds
Later Eurasian archaic lineages, including Neanderthals and Denisovans, cannot simply be folded into the recent expansion of modern humans as though all were the same population moving at the same time.Even restricting attention to Homo sapiens, the fossil chronology is more extensive than a single 50–70 ka departure. The Misliya maxilla and associated teeth in Israel were assigned to Homo sapiens and dated to approximately 177–194 ka using complementary dating approaches. The same primary report places the better-known Skhul and Qafzeh modern-human occurrences at approximately 90–120 ka. [ref]
The earliest modern humans outside Africa by Israel Hershkovitz and others. Science 359, pp. 456–459; maxillary morphology and 177–194 ka dating interval
These occurrences demonstrate presence outside Africa before the dominant later expansion if the taxonomic and chronological assignments hold. They do not by themselves demonstrate uninterrupted occupation, a particular migration route through Arabia, or a large surviving genetic contribution to present-day Eurasians.Apidima adds an important but less secure claim. Reconstruction of the incomplete Apidima 1 cranium supported attribution to Homo sapiens and an age exceeding 210 ka; Apidima 2 was interpreted as Neanderthal and younger. [ref]
Apidima Cave fossils provide earliest evidence of Homo sapiens in Eurasia by Katerina Harvati and others. Nature 571, pp. 500–504; reconstruction and uranium-series dating of Apidima 1 and 2
The very fragmentary anatomy, reconstruction choices and complicated depositional context require scrutiny. An assigned minimum age is not an exact date of arrival, and a different reconstruction or taxonomic diagnosis can alter the biogeographic inference. The sensible argument for early departures therefore uses the converging set of dated remains and its uncertainty, rather than treating the oldest proposed specimen as a decisive, uncontested fact.The main evidence favouring a single principal source is genetic. Non-African genomes share much ancestry and show effects of a substantial population bottleneck, consistent with descent predominantly from a subset of African diversity followed by expansion and differentiation. Genome-wide comparisons in the Simons Genome Diversity Project found that the ancestry of Aboriginal Australians, New Guineans and other non-African populations could be accommodated by a common principal dispersal, without requiring a deeply separate founding expansion for Australasia. [ref]
The Simons Genome Diversity Project: 300 genomes from 142 diverse populations by Swapan Mallick and others. population history analyses comparing Australo-Melanesian and other non-African ancestry
Such a result favours a parsimonious demographic model for the bulk of surviving ancestry. It does not observe a unique group crossing a border on one date, nor rule out movements whose descendants disappeared.Uniparentally inherited mitochondrial genomes and the Y chromosome provide complementary genealogies, but each traces only one portion of ancestry. Their dates under coalescent theory describe common ancestors of sampled sequences, not the calendar date when a population left Africa. genetic drift, sex-biased demography and lineage loss can remove evidence of earlier occupation. Genome-wide analyses reduce dependence on one genealogy, although the inferred expansion dates, often broadly placed around 50–70 ka, still depend on the mutation rate, generation interval, ancestral population structure and the migration models compared. A prolonged connected expansion can resemble one founder event in a simplified model.
There is also genetic evidence that complicates an absolute single-expansion claim. One analysis inferred a small contribution to Papuan ancestry from an earlier expansion, while still attributing the great majority of non-African ancestry to a shared later expansion. [ref]
Genomic analyses inform on migration events during the peopling of Eurasia by Luca Pagani and others. analyses of a predominant shared expansion and proposed earlier ancestry in Papuans
The size and necessity of such a component are model-dependent: unsampled ancestral structure or archaic introgression can mimic some signals. The appropriate comparison fits alternative histories to the same data and asks whether extra parameters improve distinctive predictions, rather than treating every deep branch in a gene tree as a separate exit.Archaic admixture makes the ancestry history explicitly reticulate. Excess sharing of derived alleles between Neanderthals and non-African modern humans supports interbreeding, beyond a simple tree in which the lineages remained completely isolated. [ref]
A draft sequence of the Neandertal genome by Richard E. Green and others. Science 328, pp. 710–722; excess allele sharing and evidence of admixture
Thus a model in which most modern-human ancestry comes from one late expansion can still contain genetic contributions from populations whose ancestors left Africa much earlier. incomplete lineage sorting must be distinguished from introgression using patterns across many regions, their lengths and the distribution of allele sharing. Back-migration into Africa further prevents “African” and “non-African” from being permanently sealed categories.Africa itself should not be represented as a homogeneous ancestral village. Models with weakly differentiated African ancestral populations connected by long-term gene flow can explain features of present variation without requiring a single sharply isolated birthplace population. [ref]
A weakly structured stem for human origins in Africa by Aaron P. Ragsdale and others. Nature 617, pp. 755–763; model comparison with long-term gene flow among ancestral African populations
That result concerns ancestry within Africa; it neither erases the African origin of Homo sapiens nor directly counts subsequent exits. Geographically, northern routes through the Levant and southern routes through Arabia remain testable alternatives or complements. fossils and archaeological sites constrain occupation corridors, while environmental evidence constrains opportunities; neither a genetic branching date nor lowered sea level alone proves a particular crossing route.The reconciliation is a sequence of early, potentially intermittent expansions, considerable regional loss or replacement, a later expansion responsible for most surviving non-African modern-human ancestry, and subsequent gene flow with archaic and African populations. Testing it requires directly dated remains, secure taxonomic comparisons, independent genetic samples, explicit demographic alternatives and allowance for unsampled populations. “One dominant ancestry expansion” is a much narrower and better-supported proposition than “only one movement out of Africa”; multiple movements need not imply several equally large surviving founding ancestries.
Past exam of the zoology course of the University of Cambridge 2025 Paper zl1 3 Solution by Codex 0 2026-10-20
Codex 0 2026-10-20Southern fossils have changed the geography, timing and anatomical character of mammaliaform evolution, while exposing how strongly a northern fossil record had shaped earlier expectations. Their importance is not that every southern lineage arose in the south. A dated occurrence establishes presence and a minimum age; an evolutionary origin requires an argument from phylogenetics and biogeography. Nor do modern continental outlines reproduce the connections of Gondwana.
A particularly consequential example is Ambondro mahabo, represented by a jaw fragment with lower teeth from Middle Jurassic Madagascar, approximately Ma. The teeth possess a basined heel associated with the crushing component of tribosphenic molars, which combine shearing and crushing in a single occlusal system. Its age extended the then-known record of this dental construction substantially backwards and challenged a simple northern origin inferred from better-sampled northern localities. The material nevertheless consists of a very restricted part of the animal, and the matching upper dentition was not directly observed. Assigning the entire skeleton, physiology or reproductive mode from these teeth would go beyond the evidence. [ref]
A Middle Jurassic mammal from Madagascar by John J. Flynn and others. Nature 401, pp. 57–60; Ambondro lower jaw, approximately 167 ± 2 million years old
The discovery also changed the character of the phylogenetic question. One hypothesis groups several southern forms in Australosphenida, associated with the ancestry of monotremes, and proposes that a tribosphenic-like construction arose independently of northern Boreosphenida, including therians. In that interpretation a highly functional tooth arrangement is convergent evolution, not a unique certificate of therian ancestry. A competing analysis supports a single origin of tribospheny and rearranges the relationships of the relevant southern taxa. [ref]
Dual origin of tribosphenic mammals by Zhe-Xi Luo and others. Nature 409, pp. 53–57; alternative placements of southern tribosphenic mammals
[ref]The evolution of tribospheny and the antiquity of mammalian clades by Michael O. Woodburne and others. phylogenetic analysis supporting a single origin of tribospheny
The important lesson is not to declare one historical topology established by the striking tooth alone. The choice depends on which cusps and basins are judged instances of biological homology, character coding, inclusion of other anatomical regions, and the taxon sample. Nor does a Middle Jurassic tribosphenic tooth by itself date the split between living marsupials and placental mammals.South American monotreme material further undermined the equation of present distribution with evolutionary birthplace. Early Paleocene Monotrematum, approximately 60–65 Ma, has teeth with affinities to the platypus lineage. Living monotremes are restricted to Australasia, but that restriction cannot be projected unchanged into the past. [ref]
First discovery of monotremes in South America by Rosendo Pascual and others. Nature 356, pp. 704–706; Paleocene Monotrematum teeth
South America, Antarctica and Australia offered changing opportunities for connection, fragmentation and movement. A South American occurrence is compatible with a geographically extensive southern history; it does not uniquely establish the direction of dispersal or prove that Monotrematum was the direct ancestor of the living platypus. The distinction between a crown group and related members of its stem group is essential when attaching such fossils to divergence-time estimates.Latest Cretaceous Madagascar has contributed more than isolated tooth surprises. The cranium of Vintana, around 70 Ma, supplied extensive new characters for the formerly tooth-dominated Gondwanatheria. Its robust feeding apparatus and unusual cranial combination permit tests of relationships and ecology that were unavailable from a few teeth. Yet a mosaic of familiar and unusual features is precisely the situation in which a single apparently diagnostic character can mislead. The placement of gondwanatherians therefore needs broad anatomical and taxonomic comparison, including other extinct groups, rather than assignment to a living order by superficial resemblance. [ref]
First cranial remains of a gondwanatherian mammal reveal remarkable mosaicism by David W. Krause and others. Nature 515, pp. 512–517; Vintana cranium and phylogenetic character sampling
The approximately 66 Ma skeleton of Adalatherium expanded that evidence into the postcranial skeleton. It documents a relatively large, several-kilogram non-therian mammal with an unusual combination of cranial, dental, vertebral and limb features. This contradicts the caricature that all Mesozoic mammaliaforms were anatomically interchangeable tiny insect-eaters. Madagascar's long isolation provides a plausible context for its evolutionary distinctiveness, but the claim that isolation caused a particular feature remains an explanatory hypothesis. One needs comparative island and continental samples to distinguish an island effect from inherited lineage-specific anatomy. [ref]
Skeleton of a Cretaceous mammal from Madagascar reflects long-term insularity by David W. Krause and others. Nature 581, pp. 421–427; Adalatherium skeleton and insularity hypothesis
Australia's early Eocene Djarthia, approximately 55 Ma, addresses a different issue: the relationships and movement of marsupials. Its ankle material supports a position close to the base of Australidelphia, a group containing the living Australian orders and the South American Microbiotheria. This is stronger evidence than assuming that every small Australian jaw belongs inside a modern Australian family. [ref]
Australia's Oldest Marsupial Fossils and their Biogeographical Implications by Robin M. D. Beck and others. PLoS ONE 3, e1858; Djarthia tarsals and australidelphian relationships
It is compatible with a history involving South America and Antarctica, but a branching order is not a map of a single migration. An extinct distribution can be extensive, intermediate populations can disappear, and the oldest sampled fossil need not occur near the place where a lineage originated. Also, the older and more inclusive Metatheria must not be confused with the living marsupial crown group.Together these discoveries change how large-scale history is tested. First, expanding southern sampling can overturn a supposed absence that arose from collecting intensity, exposure of suitable rocks or preservation. taphonomy and the concentration of many early records on durable teeth must be modelled before comparing continental diversity. Second, new skeletons can change the inferred phylogenetic tree, and therefore whether a tooth adaptation counts as one origin or several. Third, fossil calibration constrains the minimum age of a lineage, with explicit uncertainty in both geological age and phylogenetic assignment. Fourth, continental drift changes which dispersal routes were physically plausible. Shared distributions across former Gondwana may reflect vicariance, later dispersal, or a mixture; the geological separation must be compared with a defensible lineage age rather than used as its automatic explanation.
From the Jurassic through the Palaeogene, these independent discoveries have cumulatively changed both the anatomical evidence and its interpretation. They reveal a more diverse southern mammaliaform history and force explicit tests of convergence, missing data and geographic sampling, rather than replacing an assumed northern centre with an equally assumed southern centre.
Past exam of the zoology course of the University of Cambridge 2025 Paper zl1 2 Solution by Codex 0 2026-10-20
Codex 0 2026-10-20Repeated dietary adaptations reflect recurring mechanical and digestive demands, but a similar diet need not produce identical anatomy, and anatomical resemblance need not represent an independent evolutionary origin. A useful comparison places each example on a phylogenetic tree, identifies the inherited structure being modified, and separates food acquisition, oral processing and digestion.
Among dental adaptations, shearing blades recur in meat-eating mammals. In Carnivora, a placental order within Laurasiatheria, the main carnassial pair comprises the upper fourth premolar and lower first molar. Their opposing blades slice flesh, while relative development of crushing surfaces varies with diet. Predatory marsupials, including the extinct thylacine within Dasyuromorphia, also emphasize shearing, but do not reproduce precisely the same specialized tooth pair. The jaw and basic tooth classes are inherited mammalian structures; the highly blade-like feeding apparatus represents convergent evolution of performance in separate therian branches. Within Carnivora, resemblance between close relatives may instead reflect shared ancestry, and specialized insect-eating or plant-eating members demonstrate that membership of the order does not establish a carnivorous diet.
Repeated elaboration of grinding surfaces provides a complementary case. lophodonty joins tooth cusps into ridges, and selenodonty produces crescentic ridges, maintaining effective cutting edges as the surface wears. Herbivorous perissodactyls, including horses, contrast with ruminants such as bovids and cervids in Artiodactyla; both are within Laurasiatheria. Complex grinding teeth also evolved in proboscideans within Afrotheria and in macropods, a marsupial lineage within Diprotodontia. These positions rule out treating every complex herbivore tooth as one recent innovation inherited from a common grazing ancestor. Three-dimensional measurements of occlusal surface complexity in carnivorans and rodents show that dietary demands can produce comparable patterns across very different tooth constructions. The useful prediction concerns functional surface geometry, not identical cusp names in every group. [ref]
High-level similarity of dentitions in carnivorans and rodents by Alistair R. Evans and others. Nature 445, pp. 78–81; three-dimensional occlusal complexity and diet
Resistance to abrasion repeatedly modifies tooth growth as well as tooth shape. hypsodonty supplies a tall reserve crown that is progressively exposed by wear; it occurs in several ungulate groups and in some marsupials. It differs from hypselodonty, in which teeth continue growing, as in rodent incisors. Self-sharpening incisors, with uneven distribution of tooth enamel and differential wear of dental tissues, facilitate gnawing. Rodentia and Lagomorpha are both within Glires, so their incisor similarities must be analysed against that relationship rather than automatically counted as two independent origins of the whole dental system.
A high crown is a wear-management adaptation, not an infallible grass detector. Abrasive particles can come from vegetation or ingested external dust and grit; food toughness and abrasiveness are also distinct. North American horse fossils show substantial variation in dental mesowear within populations and temporal relationships between dietary abrasion and crown-height changes that are more complicated than an instantaneous switch from browsing to grazing. [ref]
Dietary Change and Evolution of Horses in North America by Matthew C. Mihlbachler and others. Science 331, pp. 1178–1181; mesowear compared with crown-height evolution
A defensible palaeodiet reconstruction combines tooth form with dental microwear, dental mesowear, stable isotope analysis where suitable, and environmental evidence. dental microwear emphasizes relatively recent meals, whereas crown form reflects inherited morphology across generations. Disagreement can therefore be informative rather than an analytical failure.A major non-dental recurrence is an enlarged gut compartment supporting microbial fermentation. mammals do not obtain the full energy value of structural plant carbohydrates through their own enzymes alone; microbial partners release usable fermentation products, notably short-chain fatty acids. foregut fermentation evolved in ruminants, colobine monkeys within Primates, and macropods. The forestomach compartments are not identical organs merely because each houses microbial digestion: the relevant independent changes concern enlargement, compartmentalization, retention and mixing in phylogenetically separated lineages. In ruminants, rumination additionally returns food for further mastication, increasing the surface available to microorganisms.
hindgut fermentation provides another solution. horses, within Perissodactyla, use enlarged caecal and colonic compartments; rabbits, within Lagomorpha, combine caecal processing with cecotrophy, reingesting selected soft material and thereby recovering microbial nutrients through a second passage. foregut fermentation allows microbial products and microbial biomass to encounter later digestive regions, whereas hindgut fermentation can accommodate high intake and rapid passage of some food fractions. Neither arrangement is universally superior: retention time, food quality, body size, intake rate and the ability to select particles affect the balance. The comparative explanation of equid success therefore requires throughput as well as percentage extraction from a single meal. [ref]
The evolutionary strategy of the Equidae and the origins of rumen and cecal digestion by Christine M. Janis. Evolution 30, pp. 757–774; retention, throughput and digestive strategies
Food acquisition supplies a further non-dental example. anteaters, within Xenarthra, and pangolins, within Pholidota in Laurasiatheria, independently combine reduction or loss of teeth with an elongated, protrusible tongue and a feeding apparatus suited to taking small social insects. Powerful forelimbs and claws can open nests, but digging also serves many other functions; claws alone do not identify ant feeding. Conversely, absence of grinding teeth need not signify nutritional simplicity: prey capture, protection from prey defences and microbial digestion can remain specialized.
Comparative dissection of primate digestive tracts supplies an independent anatomical test: gut compartments and their relative dimensions can be compared with diet rather than guessed from the teeth. Such comparisons must account for body size and the non-independence of related taxa. [ref]
Morphology of the gastrointestinal tract in primates: comparisons with other mammals in relation to diet by David J. Chivers and others. Journal of Morphology 166, pp. 337–386; comparative gut measurements and dietary categories
Testing these interpretations requires more than a gallery of look-alikes. Record diet in wild animals, compare anatomical performance under relevant loads, measure gut retention or digestive products, and include relatives with different diets. Control for body size, age, sex, tooth wear stage and shared ancestry, since ten related grazers are not ten independent evolutionary experiments. For fossils, preserve the distinction between direct anatomical observation and an inferred gut or behaviour. The repeated solutions are cutting or grinding surfaces, mechanisms that sustain those surfaces under wear, specialized acquisition structures and microbial digestive chambers; their phylogenetic distribution reveals both convergence and inherited constraints. Past exam of the zoology course of the University of Cambridge 2025 Paper zl1 1 Solution by Codex 0 2026-10-20
Codex 0 2026-10-20cetaceans illustrate a sequence of inherited mammalian features, terrestrial specializations and subsequent aquatic transformations, followed by divergence in feeding and sensory anatomy. This is a branching phylogenetic tree, not a procession of named fossils that can all be identified as direct ancestors. Here Cetacea includes living whales, dolphins and porpoises; mammals means the crown group containing living monotremes and therians, whereas mammaliaforms also includes close extinct relatives outside that crown group. Dates below are approximate millions of years ago, abbreviated Ma.
The starting condition is a terrestrial, non-mammaliaform cynodont, itself a therapsid within Synapsida. Along the mammalian stem group, enlargement of the dentary and reduction of the other lower-jaw bones accompanied more differentiated teeth, increasingly precise dental occlusion and elaboration of a secondary palate. These changes belong to a feeding and respiratory complex: a larger tooth-bearing bone carries the mastication load, differentiated teeth process food, and a bony partition separates nasal and oral passages. They were acquired in a mosaic; neither a full modern mammalian jaw nor the aquatic body plan appeared at the initial divergence from other cynodonts.
Early mammaliaforms show how jaw support and hearing became reorganized. Morganucodon, around the Triassic–Jurassic transition and Early Jurassic, retained the old articular–quadrate jaw joint alongside a dentary–squamosal joint. In the mammalian condition the dentary–squamosal articulation supports the jaw, while the articular and quadrate correspond to the malleus and incus; the angular bone contributes to the ectotympanic. This is biological homology supported by comparative anatomy and biological development, not merely similarity in function. Hadrocodium, about 195 Ma, records further changes in jaw attachment and the braincase consistent with increased separation of mastication and hearing. Its tiny skull does not preserve an entire living-style ear apparatus; the reconstruction depends partly on bony attachment evidence. [ref]
The inherited mammalian package also includes diphyodonty, hair and lactation, although the latter two leave much poorer evidence in these particular fossils than do teeth and jaws. Precise adult dental occlusion is easier to maintain when repeated replacement ceases. The lineage subsequently passed through Theria, Eutheria and the ancestors of living placental mammals. These nested relationships matter: a Cretaceous eutherian is not automatically a member of the living placental crown group, and neither the first known fossil nor the date of a tooth innovation fixes the origin of an entire group.
The immediate terrestrial context of whale evolution is within Artiodactyla, broadly circumscribed to include Cetacea. Living hippopotamuses are the closest living relatives of cetaceans, not their ancestors. Some early whale teeth suggested relationships with extinct mesonychians, but dental resemblance alone was misleading. Early whale skeletons preserve the characteristic artiodactyl double-pulley astragalus, providing a powerful independent anatomical test of the relationship inferred from molecular evidence. The relevant comparison is the detailed construction of the ankle, not simply whether an animal has hooves or eats meat. [ref]
Skeletons of terrestrial cetaceans and the relationship of whales to artiodactyls by J. G. M. Thewissen and others. Nature 413, pp. 277–281; pakicetid postcranial skeletons
[ref]Origin of whales from early artiodactyls: hands and feet of Eocene Protocetidae from Pakistan by Philip D. Gingerich and others. Science 293, pp. 2239–2242; protocetid ankle anatomy
Early Eocene pakicetids, roughly 50 Ma, combine a largely terrestrial, weight-bearing skeleton with diagnostic whale ear-region anatomy, notably the thickened medial wall of the auditory bulla called the involucrum. Thus identification as a whale does not imply an obligately marine animal. Ambulocetus, roughly 48 Ma, has a different combination: robust limbs still useful around shore, large feet and an axial skeleton suited to substantial movement in water. Reconstruction of amphibious locomotion uses limb proportions, joint surfaces and vertebral anatomy together; it does not require assuming that its swimming exactly resembled an otter's. These are successive grades represented by branching relatives, not proof that a particular pakicetid gave birth to the known Ambulocetus specimen. [ref]
From Land to Water: the Origin of Whales, Dolphins, and Porpoises by J. G. M. Thewissen and others. sections on pakicetids, ambulocetids, protocetids and basilosaurids
Middle Eocene protocetids further document reduction of terrestrial support and increasing commitment to swimming. Changes in the connection between pelvis and vertebral column, limb proportions and the position of external nostrils occurred in different combinations. The ankle of Rodhocetus is especially informative about ancestry even while other parts of its skeleton document aquatic specialization. It would be unjustified to draw a preserved tail fluke onto Rodhocetus: a reconstructed swimming mode must distinguish actual preserved anatomy from inferred soft parts. [ref]
Origin of whales from early artiodactyls: hands and feet of Eocene Protocetidae from Pakistan by Philip D. Gingerich and others. Science 293, pp. 2239–2242; protocetid ankle anatomy
Aquatic hearing changed alongside locomotion. Enlargement of the mandibular sound-reception region and changes in the middle ear support a transition towards receiving underwater sound through the lower jaw, with increasing acoustic separation of the ears from the skull. Early whale lineages display different intermediate combinations, so the presence of an involucrum alone does not imply a modern dolphin hearing system. Reconstructing soft sound-conducting tissues requires comparison with living anatomy; the fossil preserves their bony context rather than the entire pathway. [ref]
Eocene evolution of whale hearing by Sirpa Nummela and others. Nature 430, pp. 776–778; sound transmission reconstructed from early whale ear and jaw anatomy
By the later Eocene, basilosaurids were fully aquatic. The forelimbs functioned as flippers, the vertebral column and tail supplied propulsion, and the hind limbs were far too small to support terrestrial walking. Nevertheless, the reduced limbs of Basilosaurus retain recognizable limb and foot elements. Loss of a locomotor role is not equivalent to absence of all function; reproductive or muscular roles are compatible with reduction, although a specific behaviour cannot be read directly from a bone. The transition therefore involved changing proportions and connections as well as losses. [ref]
Hind limbs of Eocene Basilosaurus: evidence of feet in whales by Philip D. Gingerich and others. Science 249, pp. 154–157; reduced pelvis and hind limbs
Finally, the living branches acquired different specializations. Odontoceti retain teeth and evolved specialized sound production and echolocation; Mysticeti evolved baleen and lack functional adult teeth. fossil toothed mysticetes and degraded enamel-related genes show that modern toothlessness is derived. Palatal vascular features have been used to infer an intermediate combination of teeth and baleen, but such foramina do not preserve the baleen itself, and the exact sequence of feeding behaviours is less secure than the transition from toothed ancestry. [ref]
Morphological and molecular evidence for a stepwise evolutionary transition from teeth to baleen in mysticete whales by Thomas A. Deméré and others. Systematic Biology 57, pp. 15–37; palatal foramina, tooth characters and enamel-gene pseudogenes
The resulting history explains why a whale can have a mammalian jaw and reproductive system, an artiodactyl ancestry, a radically modified swimming skeleton, and a feeding apparatus that evolved after the aquatic transition. The strongest reconstruction combines nested anatomical characters with independently dated fossils, while treating soft-tissue and behavioural reconstructions as hypotheses. Past exam of the zoology course of the University of Cambridge 2024 Paper ZM5 6 Solution by Codex 0 2026-10-20
Codex 0 2026-10-20The mirror-mark test can provide evidence that an animal uses reflected information to identify and act on its own body. It is a narrower assay than a general test of self-awareness, and failure is especially difficult to interpret. The core inference rests on directing an action to the otherwise unseen marked body part, rather than merely responding to something unusual in a mirror.
In a suitable design, an animal first has opportunities to inspect a mirror without a mark. A visible mark is then placed where it cannot be seen directly, using a procedure that avoids an informative tactile, olfactory or handling cue. After recovery from any necessary handling, investigators compare responses with the mirror available and unavailable, and with a matched invisible sham treatment. The predicted response is mark-directed investigation of the animal's own body specifically when the visible change can be seen in reflection. Looking at the mirror, attacking it or searching behind it are interesting observations, but do not alone establish bodily self-recognition.
The classic chimpanzee study used prior mirror exposure and otherwise unseen dye marks to demonstrate self-directed investigation. [ref]
Chimpanzees: Self-Recognition by Gordon G. Gallup Jr.. Science 167, pp. 86–87; mirror exposure, hidden dye marks and self-directed touching
Its conceptual advance was to turn a claim about self-recognition into a behavioural prediction that could be compared with alternative responses. A mark on the reflected forehead corresponds to a location on the subject's own forehead. Reaching there uses information about the relation between the image and body; trying to touch the glass instead supports a different interpretation. An odourless mark that is imperceptible by touch makes this distinction stronger.A rigorous modern design makes those alternatives explicit. In a factorial comparison, let and denote rates of appropriately localized body-directed actions for visible and sham marks with a mirror, and let and denote the corresponding rates with the mirror covered. The interaction contrast:asks whether the visible mark's effect specifically depends on reflective information. A positive is useful only if the actions are correctly localized, opportunities to act are comparable and uncertainty is estimated across animals. It does not acquire a cognitive interpretation just because its statistical test is significant. General increases in grooming, attention or agitation need to be coded separately.
Controls should match application pressure, odour, texture and handling, vary mark side or location, and counterbalance condition order. A covered mirror controls its physical presence; a live or recorded other animal helps characterize social responses. Noncontingent or delayed self-images can test the importance of immediate sensorimotor contingency, though they also increase task difficulty. Separate trials with directly visible marks help establish that a subject notices such a change and has an available response, without training the critical hidden-mark action in advance. Coders should be blinded where feasible, and the criteria for a pass specified before viewing the outcome. Repeated touches by one animal are not independent evidence from many animals.
A positive result supports at least a learned mapping between reflected information and the subject's body. How much more it supports is a problem of construct validity. An animal might combine visual contingencies, proprioception and a body schema without representing itself as a named, temporally continuous individual. Conversely, learning the mapping does not make the result meaningless: learned information about one's own body can itself be a form of self-representation. The question is which alternative mechanisms the design distinguishes. A pass does not by itself demonstrate theory of mind, autobiographical memory, moral understanding or a particular subjective experience.
Negative results are weaker because successful performance requires several capacities together: noticing the mark, attending to reflection, relating the image to the body, being motivated to investigate, and possessing a suitable action. Fear, social attraction to the image, poor visual access or indifference to marks can prevent the predicted response even when some self-related information is available. ecological validity is therefore central. Mirror dimensions, access, viewing geometry and prior experience must suit the species. Uniformly presenting a small mirror to animals of very different sizes does not create a biologically equivalent test.
The elephant study illustrates this dependence. Three asian elephants were exposed to a large accessible mirror and visible and sham marks. One passed the mark criterion, while the others also showed informative mirror-oriented exploration. [ref]
Self-recognition in an Asian elephant by Joshua M. Plotnik and others. PNAS 103, pp. 17053–17057; large accessible mirror, visible and sham marks, one of three subjects passing
This is evidence about the observed individuals and assay, not a species-wide estimate based on one success, nor proof that the nonpassing individuals lacked every form of self-representation. The apparatus enabled close physical exploration that smaller or inaccessible mirrors would not permit.The required action must also reflect anatomy. Bottlenose dolphins cannot use a hand to touch a facial mark. Investigators therefore examined orientations and movements exposing marked regions to a reflective surface, comparing marked and sham-marked conditions. [ref]
Mirror self-recognition in the bottlenose dolphin: A case of cognitive convergence by Diana Reiss and Lori Marino. PNAS 98, pp. 5937–5942; marked and sham-marked dolphins and mirror-oriented body inspection
Such an adaptation avoids treating hand use as a cognitive prerequisite, but creates a greater interpretive burden: body inspection must be distinguished from ordinary swimming, attention to handling or generalized interest in the mirror. Spatially specific changes and blinded coding are particularly valuable.cleaner wrasse challenge assumptions about which animals should count as passing. Following mirror exposure, fish with coloured marks on otherwise unseen regions scraped their bodies in the mirror condition; transparent marks and coloured marks without a mirror did not elicit the same pattern. [ref]
If a fish can pass the mark test, what are the implications for consciousness and self-awareness testing in animals? by Masanori Kohda and others. PLoS Biology 17, e3000021; cleaner wrasse, coloured versus transparent marks and mirror-dependent scraping
The ecological relevance of parasite-like marks helps explain motivation and sharpens the test. It also raises mechanistic questions about whether the animal identifies a persistent visual self or uses learned reflected cues to localize a possible parasite. Those alternatives require further controls and transfer tests; accepting a behavioural criterion in mammals but rejecting identical criteria solely because the animal is a fish would be inconsistent.Tests in other modalities can help identify capacities missed by a visual assay. dogs investigated modified own odours more than unmodified own odours, with comparisons involving other dogs and the added odour alone. [ref]
Smelling themselves: Dogs investigate their own odours longer when modified in an “olfactory mirror” test by Alexandra Horowitz. Behavioural Processes 143, pp. 17–24; own, modified-own, other-dog and modifier-only odour comparisons
The modifier-only comparison addresses simple interest in a novel smell, but sniffing longer does not require locating a change on one's own body. It consequently supports odour discrimination and a possible self-related comparison more directly than it establishes the same representation tested by hidden-mark localization. Ecologically appropriate tasks should be compared in terms of their information and inferential demands, rather than all being declared interchangeable mirror tests.A stronger account would combine spontaneous mirror-guided inspection, transfer to new untrained body locations or viewing arrangements, and independent tasks probing self-related information. Training should be reported explicitly: success after reinforcement demonstrates a learned capacity under those conditions, while spontaneous generalization supports a different claim. Samples should include individual and developmental variation, and comparative analyses should retain uncertainty rather than coding entire species as cognitively present or absent after a handful of observations.
A well-controlled pass is evidence for mirror-guided bodily identification; it is not a complete measure of a self-concept. A failure is compatible with absent capacity, unsuitable task demands or insufficient motivation. The mirror-mark test is most useful as one component of a comparative research programme that separates those possibilities.
Past exam of the zoology course of the University of Cambridge 2024 Paper ZM5 5 Solution by Codex 0 2026-10-20
Codex 0 2026-10-20The proposed asymmetry is not generally defensible: animal behaviour and immunity form a reciprocal system, and “more” has no common meaning without an outcome, scale and intervention. Avoiding infection, controlling pathogen growth, tolerating tissue damage and changing social contact are different outcomes. Their causal effect sizes cannot be ranked by counting examples in either direction.
The definition of immunity matters first. In its narrower physiological sense, it concerns cellular and molecular defences. A behavioural immune system describes actions that reduce exposure before those defences are challenged, while social immunity includes protection generated by interactions among group members. If avoidance is defined as part of immunity, a statement that animal behaviour influences immunity becomes partly true by definition. A useful analysis instead specifies whether an action changes exposure, immune activity, pathogen burden or the damage associated with that burden. disease resistance reduces burden; disease tolerance reduces damage at a given burden. Lower illness alone does not distinguish these routes.
One strong route from animal behaviour to defence is the management of exposure. Choice of food, mates and social partners determines contact with infectious material. grooming can remove external parasites, and hygienic behaviour can remove contaminated material from a nest. Conversely, aggregation and some forms of close social contact can increase opportunities for transmission. These effects depend on the pathogen's transmission route: removing one kind of contact need not reduce infection spread by an environmental reservoir. An observed association between sociability and infection can also arise because infection changes sociability, making temporal or experimental evidence essential.
honeybee colonies selected for hygienic behaviour provide a causal evolutionary and experimental example. Selection based on brood-removal assays was combined with exposure to American foulbrood disease, allowing disease outcomes in selected and comparison colonies to be assessed. Removal of infected brood can reduce a colony's infectious reservoir and protect other individuals. [ref]
Resistance to American foulbrood disease by honey bee colonies Apis mellifera bred for hygienic behavior by Marla Spivak and Gary S. Reuter. Apidologie 32, pp. 555–565; selected hygienic colonies, brood assays and pathogen challenge
The result concerns colony protection, not a demonstration that each worker's cellular immunity is stronger. Selection can change correlated traits as well as brood removal, so a mechanistic follow-up should match colony size, brood age, exposure and background, and manipulate the opportunity for removal. Colonies are independent experimental units; scoring many cells within one colony does not create many independently selected colonies.Choice of an offspring’s food plant can also change the chemical environment encountered by parasites. Infected monarch butterflies preferentially laid eggs on plants that reduced parasite growth and disease in their offspring. This supported transgenerational medication: neither a simple cure of the mother nor merely a demonstration that a toxic plant can inhibit a parasite. [ref]
Evidence for trans-generational medication in nature by Thierry Lefèvre and others. Ecology Letters 13, pp. 1485–1493; infected monarch mothers, oviposition choice and offspring parasite growth
The inference needs both the infection-dependent change in oviposition and the offspring benefit. Tests should include infected and uninfected mothers offered the same plant alternatives, standardized parasite exposure of offspring, and measurements of larval growth and survival as well as parasite burden. Nutritional quality and general plant preference are competing explanations. A cost of the medicinal plant in parasite-free conditions would additionally help explain why every individual does not always choose it.animal behaviour can influence physiological immunity as well as exposure. Activity, feeding and sleep affect resource acquisition and allocation, while social interactions can alter endocrine and neural signals. These are plausible routes, but a study must measure the relevant immune process and not infer it from survival alone. An immune assay can increase because the animal is more infected, rather than because it has greater protective capacity. randomization, controlled nutrition and repeated observations can help separate these interpretations. Any claim of a trade-off should identify the limiting resource and the competing biological fitness demands; a change in one circulating marker is insufficient.
The reverse direction is equally substantive. Immune challenges can change activity, appetite, social investigation and priorities, producing sickness behaviour. Such changes may conserve resources, reduce exposure to further hazards or alter transmission, but some can instead reflect damaging inflammation or a pathogen's manipulation. Reduced activity after infection is therefore not automatically adaptive host defence. Comparing host biological fitness with and without the response, and separating immune activation from direct pathogen action, is necessary for an evolutionary interpretation.
lipopolysaccharide provides one experimental way to induce an inflammatory response without a replicating pathogen. Work on lactating house mice showed that the resulting effects depended on the activity and environmental context: pup retrieval could be maintained, and cold conditions elicited nest building despite the challenge. [ref]
Differential Effects of Lipopolysaccharide on Pup Retrieving and Nest Building in Lactating Mice by Arnaud Aubert and others. Brain, Behavior, and Immunity 11, pp. 107–118; immune challenge, maternal behaviour and ambient temperature
This supports a reorganization of competing motivations rather than simple global paralysis. It does not show that all illness-related inactivity is strategic. Controls should match handling and injection, assess motor capacity and temperature, and distinguish loss of appetite from inability to acquire food. Dose and timing also matter: an artificial inflammatory challenge need not reproduce a natural infection's trajectory. Blocking a candidate immune mediator, followed by a rescue intervention, would provide stronger evidence for a specific immune-to-neural pathway than a challenge alone.Immune influences are not confined to overt sickness. In house mice, work on interferon-gamma linked immune deficiency and altered social preference to changes in neural connectivity and inhibitory physiology. Immune restoration and targeted signalling interventions strengthened a mechanistic interpretation beyond a correlation between illness and social withdrawal. [ref]
Unexpected role of interferon-γ in regulating neuronal connectivity and social behaviour by Anthony J. Filiano and others. Nature 535, pp. 425–429, Figs. 1–2; immune deficiency, IFN-γ interventions, neural physiology and social preference
The experiments support a role for immune signalling in the tested neural and behavioural context; they do not establish a universal explanation of sociability or justify extrapolating a house mouse social-preference assay directly to human psychiatric conditions. Sensory ability, general activity, anxiety-related responses, housing and genetic background remain important controls when interpreting such assays.The two directions can form the same feedback loop. An immune response changes social contact; changed contact alters subsequent exposure and infection; the new infection state changes the immune response again. The medication example similarly links infection-dependent action to offspring defence. Neither direction is an independent input fixed while the other acts. A useful factorial design would manipulate a specific action or opportunity for action and a specific immune challenge, then measure both behavioural and physiological outcomes over time. Baseline health, age, sex and reproductive state should be controlled, and the manipulation of action should avoid introducing injury or stress that independently changes immunity.
A claim that one direction is larger would require comparable interventions and a shared endpoint, such as lifetime reproductive success or pathogen transmission, with uncertainty over an explicitly chosen time horizon. Different answers may follow for individual survival, colony persistence and epidemic spread. The evidence supports bidirectional, context-dependent regulation: actions govern exposure and defence, while immune signals govern behavioural priorities and sometimes normal neural function. A universal ranking conceals precisely the causal distinctions needed to understand this system.
Past exam of the zoology course of the University of Cambridge 2024 Paper ZM5 4 Solution by Codex 0 2026-10-20
Codex 0 2026-10-20Apparent resemblance generates competing hypotheses, not a diagnosis of mimicry. Establishing receiver-relevant similarity, evolutionary history and the biological fitness effect of resemblance are separate tasks. Shared ancestry, shared developmental responses and similar ecological demands may all contribute, and the origin of a pattern need not be the same as the process currently maintaining it.
First establish that the sampled individuals represent distinct species and comparable life stages and sexes. Voucher records, repeated observations, morphology and independent genetic evidence help distinguish species from geographical forms or sexually different members of one species. Sampling should span localities, seasons and within-species variation, since choosing only strikingly similar specimens exaggerates community-wide resemblance. For each individual, record dorsal and ventral patterns, size, resting posture, flight behaviour, microhabitat and activity time. An identical-looking patch in a photograph may rarely be exposed to the same receiver in nature.
Similarity must then be measured for plausible receivers. Predatory birds and butterfly mates need not share human colour vision. Calibrated reflectance measurements across visible and ultraviolet wavelengths, natural illumination and relevant backgrounds can support a colour vision model. A simplified relative receptor quantum catch is:where is illumination, surface reflectance and the effective spectral sensitivity of receptor class . The comparison should include receptor noise and spatial resolution, because two spectrally distinguishable patches may be unresolved at attack distance. An apparent human match may conceal an ultraviolet or spatial difference. Conversely, experimentally demonstrated predator generalization can establish functional similarity despite a difference obvious to a human. A model predicts discrimination; behavioural tests verify whether the animal actually uses it.
One hypothesis is retention of an ancestral pattern through biological homology. Infer relationships from many independent genomic regions, then reconstruct pattern changes with uncertainty on the resulting phylogenetic tree. Resemblance concentrated among close relatives is compatible with retention. Similarity among distant relatives, especially matching different local patterns in different places, supports repeated change, although uncertainty in ancestral states must be retained. A single wing-pattern gene tree cannot serve as the independent species history when that very region might have crossed species boundaries.
A second hypothesis is Müllerian mimicry. If several species are defended and share predators, a common warning pattern can reduce the number of individuals attacked while predators learn avoidance. A local mimicry ring is predicted, with newcomers to an unfamiliar pattern suffering more attacks. Measure defence rather than infer it from colour: chemical assays, controlled feeding responses and subsequent predator behaviour address different components of palatability. predators from different localities may have different experience, so both naive and experienced receivers are informative. Several defended species can differ in defence strength; their interaction need not fit a perfectly symmetric mutual benefit.
A third hypothesis is Batesian mimicry, in which a relatively undefended species gains protection by resembling a defended model. This predicts protection dependent on the model's presence, abundance and the receiver's experience. A resemblance experiment should therefore vary both visual matching and the frequency or density of defended and undefended prey. A palatable mimic that becomes too common can weaken learned avoidance, whereas sharing a well-defended signal can reinforce it. These are ecological predictions to test, not a rule that each natural assemblage falls into one simple category. Defence varies with diet, age and the predator used in the assay.
The critical causal experiment changes the signal while controlling the rest of the prey. Artificial prey or wing models can independently vary colour and geometry against a standardized food reward. Randomized placement and position changes control background and location; handling and paint controls are needed with live butterflies. Record detection, attack and rejection separately: fewer missing prey can reflect poor detection rather than avoidance after recognition. Camera records help identify actual predators and distinguish attack from weather damage or removal by other animals. Artificial models lack movement and some chemical information, so their results should be checked against observations of live prey where feasible.
A field precedent is the release of different Heliconius cydno colour morphs into communities with different abundant co-models. Survival patterns supported an advantage to local matching, and the experiment also examined the prediction that this disadvantage should decrease with increased release density. [ref]
Three-butterfly system provides a field test of müllerian mimicry by Durrell D. Kapan. Nature 409, pp. 338–340; H. cydno release experiments, local co-models and release density
This is more informative than simply mapping similar butterflies in the same forest. However, disappearance after release can include dispersal and unequal detectability; recapture effort, movement observations and attack evidence are needed when adapting such a design. Replication belongs at the site or independently manipulated community level, rather than treating every observation within one site as an independent community comparison.Other ecological explanations deserve distinct predictions. Shared crypsis could make species match the same leaves, bark or light environment without resembling one another as defended models. Test detection against matched and mismatched backgrounds, separating the visibility of the prey from a predator's willingness to consume it. Shared thermoregulatory demands could favour similar absorption properties; temperature and performance measurements would then be relevant. Similar mate-detection environments could favour similar signals, but mate preference experiments must establish the relevant receiver and show how species avoid reproductive confusion. These mechanisms can coexist with defensive mimicry.
A common developmental or environmental cause is another possibility. Rear offspring from different populations and species in standardized and experimentally varied conditions, controlling larval diet, temperature and age. Persistence of differences under common rearing supports inherited contributions; condition-dependent convergence supports phenotypic plasticity. Crosses and quantitative trait locus mapping can then test the genetic architecture of patterning. Work on Optix in Heliconius combined mapping, expression and population comparisons to identify a shared regulator of red wing patterning. [ref]
optix Drives the Repeated Convergent Evolution of Butterfly Wing Pattern Mimicry by Robert D. Reed and others. Science 333, pp. 1137–1141; mapping, expression and population genetics of red wing patterning
Use of the same developmental gene does not by itself prove a single recent origin of the pattern, nor prove that resemblance is adaptive.Finally, adaptive introgression could transfer a pattern-associated region between species. Genome-wide ancestry should be compared with local ancestry around pattern regions, testing alternatives such as incomplete lineage sorting. The Heliconius genome study found evidence of exchange associated with mimetic adaptations among lineages. [ref]
Butterfly genome reveals promiscuous exchange of mimicry adaptations among species by The Heliconius Genome Consortium. Nature 487, pp. 94–98; genomic comparisons and introgression around mimicry loci
This concerns the route by which a useful pattern is acquired; selection by predators can still explain its maintenance. The strongest explanation combines receiver-specific similarity, a tested ecological benefit and an independently supported developmental and evolutionary history; neither human resemblance nor a shared pattern-associated gene supplies all three. Past exam of the zoology course of the University of Cambridge 2024 Paper ZM5 3 Solution by Codex 0 2026-10-20
Codex 0 2026-10-20Knowing the molecular basis of a behaviour is not a prerequisite for understanding its evolution or many of its evolutionary consequences. Evidence about transmission is essential for claims of inherited change, while detailed genetic architecture becomes essential for particular mechanistic predictions. The claim therefore depends on what is meant by a genetic basis and on the explanatory question being asked.
Tinbergen's four questions distinguish mechanism, development, adaptive significance and evolutionary history. Identifying a neural or molecular mechanism helps explain how a response is produced; it does not automatically show why a variant spread, whether it currently increases reproductive success, or whether the same mechanism generated the ancestral transition. Conversely, a well-supported evolutionary explanation can begin with experimentally demonstrated biological fitness consequences and transmission without a complete molecular account. These explanatory levels are complementary rather than substitutes. [ref]
On aims and methods of Ethology by Nikolaas Tinbergen. Zeitschrift für Tierpsychologie 20, pp. 410–433; causation, development, survival value and evolution
The phrase genetic basis can refer to several different achievements: identifying inherited variation; estimating the number and effects of contributing genetic loci; finding a causal nucleotide change; or describing every gene required for development of the relevant sensory and motor systems. These are not equivalent. Many genes can be necessary for an animal to perform an action while none explains variation in that action within the studied population. Knocking out a broadly required neural gene and eliminating courtship does not identify an evolutionary substitution for a naturally varying mate preference.
quantitative genetics can predict a response without naming the causal molecular variants. Under the appropriate additive, generational and environmental assumptions, the multivariate breeder's equation gives:where is the additive genetic covariance matrix and the vector of phenotypic selection gradients. Behavioural measurements, pedigrees, repeated observations and reproductive success can therefore estimate whether and in what direction a response is expected. The covariances matter: selection favouring exploration can produce a correlated response in aggression or constrain the response when their biological fitness effects conflict. Naming an exploration-related gene would not replace this population-level information.
These estimates require strong controls. behavioural repeatability is consistency among observations of the same individual; it can reflect persistent environment as well as inherited differences and is not equivalent to heritability. Parent–offspring resemblance can also reflect teaching, maternal provisioning or shared habitat. cross-fostering, common garden experiments and appropriately structured breeding designs help separate these alternatives. heritability is conditional on the sampled population and environment, not a measure of immutability. A response measured in one environment may fail elsewhere because of genotype-environment interaction or altered selection. Thus ignorance of exact molecular variants is compatible with informative prediction, but ignorance of transmission and its confounders is not.
Molecular work adds power when it establishes a causal link to naturally occurring variation. In Drosophila melanogaster, rover and sitter food-search variants were connected to the foraging gene, which encodes a cGMP-dependent protein kinase. Mapping, enzyme activity and transgenic rescue linked the molecular difference to behavioural performance; comparable locomotion without food helped exclude a general activity explanation. [ref]
Natural Behavior Polymorphism Due to a cGMP-Dependent Protein Kinase of Drosophila by K. A. Osborne and others. Science 277, pp. 834–836, Tables 1–3; foraging variants, kinase activity and transgenic rescue
This is much stronger than finding a statistical association between a gene and a behavioural score. Nevertheless, the experiment alone does not establish which ecological conditions historically maintained the polymorphism. That requires biological fitness comparisons across resources, densities and frequencies, with genetic-background controls.genetic architecture is particularly informative when animal behaviour changes gene flow. In Heliconius melpomene and Heliconius cydno, mapping identified several major regions associated with male mating preferences; one lay close to the wing-pattern regulator Optix. Tight genetic linkage can help maintain associations between a mating cue and preference despite exchange between lineages. It does not establish pleiotropy, and courtship assays must distinguish attraction from the female's response and subsequent mating. [ref]
Genetic dissection of assortative mating behavior by Richard M. Merrill and others. PLoS Biology 17, e2005902; preference QTLs, linkage to optix, and limitations of courtship assays
Here molecular localization helps evaluate whether a proposed route to reproductive isolation is genetically feasible. A preference could still have been shown to reduce heterospecific mating before its contributing regions were mapped.The influence of one individual's animal behaviour on another's development further complicates a simple own-genotype explanation. Maternal provisioning in Onthophagus taurus was studied using a breeding design that separated direct and maternal genetic contributions to offspring traits. [ref]
The genetics of maternal care: direct and indirect genetic effects on phenotype in the dung beetle Onthophagus taurus by John Hunt and others. PNAS 99, pp. 6828–6832; paternal half-sib design, brood mass and maternal contributions
An indirect genetic effect occurs when another individual's inherited properties alter the focal individual's phenotype. Such effects change the environment in which selection acts and can alter expected evolutionary responses. Identifying only the offspring's molecular variants would miss an important part of the causal system. Conversely, an observed maternal effect is not automatically a maternal genetic effect; provisioning can vary for environmental reasons.Transmission need not follow genetic parentage. In wild great tits, experimenters trained demonstrators to use alternative puzzle-box techniques and followed the spread of the introduced variants. Persistent local traditions and preferential adoption of the common local technique supported social learning and conformist transmission. [ref]
Experimentally induced innovations lead to persistent culture via conformity in wild birds by Lucy M. Aplin and others. Nature 518, pp. 538–541; seeded puzzle-box techniques and social diffusion in wild great tits
The experiment established a route of behavioural inheritance without identifying a molecular difference between the techniques' users. It did not prove that learning ability has no inherited basis, or that the new tradition changed allele frequencies. Rather, it shows why an account of behavioural change needs to identify the relevant transmission process instead of assuming it.Even a learned response with no demonstrated inherited differences can influence subsequent evolution. A new resource use can alter selection on digestion; a socially learned mating signal can alter assortative mating; habitat choice can change contact with other populations. The immediate causal effect can be tested by manipulating the action or its social transmission and measuring biological fitness or exchange. To claim ensuing genetic adaptation, one must additionally show inherited change. To explain exactly which variants can respond, how quickly, and with what correlated effects, information about genetic architecture becomes increasingly valuable.
The most productive programme therefore combines behavioural intervention, transmission studies, biological fitness measurement and molecular analysis when it addresses an unresolved mechanism. Candidate variants should be tested across natural genetic backgrounds and environments, preferably with targeted perturbation and rescue; historical claims also need comparative or temporal evidence. Exact molecular knowledge is neither sufficient nor universally necessary: the necessary evidence is the evidence that connects the particular behavioural difference, its transmission and its measured evolutionary consequence.
Past exam of the zoology course of the University of Cambridge 2024 Paper ZM5 2 Solution by Codex 0 2026-10-20
Codex 0 2026-10-20reinforcement is the strengthening of reproductive barriers by selection against costly hybridization. Its importance must be demonstrated causally, rather than inferred solely from greater mating discrimination where species meet. Typically, partially isolated lineages encounter one another, produce low-fitness hybrids, and experience selection favouring discrimination that reduces such matings. secondary contact after divergence is a common setting, but the definition concerns the selective mechanism rather than one obligatory geographical history.
Consider a rare inherited preference that reduces the probability of producing a hybrid by , when hybrid offspring lose a proportion of reproductive success relative to within-population offspring. In a simplified accounting with a common offspring-equivalent denominator, the benefit is . If stronger discrimination costs through delayed mating or rejection of suitable mates, it is favoured when:This expresses the logic of reinforcement, not a complete population genetics model. Encounter rates determine , sex-specific costs can differ, and gene flow, recombination and associations between preference and ancestry determine whether discrimination can evolve and persist. The mere existence of low-fitness hybrids does not guarantee that an effective preference variant is available or that its costs are small.
The first empirical requirement is evidence for contact and opportunity to hybridize. Maps should establish coexistence at the scale of mating, not merely occurrence within the same region. Field observations and parentage or genomic ancestry estimates can establish heterospecific mating and recent gene flow. Historical contact may also be relevant if successful reinforcement has already made contemporary hybrids rare. Complete present-day separation therefore does not disprove a past role, but it makes that historical role harder to identify. Models fitted to genomic data should compare alternative demographic histories rather than equating shared alleles automatically with recent introgression.
The second requirement is a reproductive cost. Reciprocal crosses should measure fertilization, survival, fertility and subsequent reproductive success, including later-generation and backcross offspring where feasible. Reduced performance may be intrinsic, such as hybrid sterility, or ecological, such as failure to use either parental habitat effectively. Laboratory survival alone can miss the latter. Reciprocal environmental comparisons with parental controls test whether hybrid disadvantages persist under natural conditions. Handling effects, parental condition and rearing density should be standardized. Selection against hybrids must be distinguished from lower mating rates caused solely by ecological separation.
The third requirement is variation in barriers consistent with selection against those costs. A classic prediction is reproductive character displacement: stronger discrimination in sympatry than in populations outside the contact zone. Female Drosophila pseudoobscura from regions shared with Drosophila persimilis showed greater sexual isolation than females from outside that overlap, providing an influential test of this prediction. [ref]
Speciation driven by natural selection in Drosophila by Mohamed A. Noor. Nature 375, pp. 674–675; geographic variation in female discrimination against D. persimilis
Comparisons should use several independent populations, matched environments and standardized male stimuli. Both choice and no-choice assays are useful: the former measures relative preference among available partners, whereas the latter asks whether rejection persists when an alternative partner is absent. Neither alone estimates realized gene flow in the field.The geographic pattern has important alternatives. Different environments can independently favour different signals or sensory responses; sexual selection within each lineage can generate divergence; existing discrimination can permit coexistence while poorly discriminating populations disappear. This last process can sort populations without increasing discrimination within them. Costly heterospecific courtship can also favour signal divergence without selection against hybrid offspring. Such reproductive interference is relevant to isolation, but should not automatically be called reinforcement in its strict hybrid-cost sense. Common garden experiments help distinguish inherited differences from immediate effects of environment or experience, but do not on their own identify the historical selective cause.
Crosses and mapping provide a further line of evidence. In the Drosophila pseudoobscura system, crosses between populations with stronger and weaker discrimination showed inherited variation in enhanced discrimination, with high discrimination expressed in first-generation crosses. Chromosome substitutions and finer mapping implicated multiple regions, and their contributions differed among sampled populations. Controls measured male mating attempts, helping separate female rejection from altered male effort. Importantly, candidate regions enriched for olfactory functions were suggestive rather than proof of a particular sensory mechanism; mapping an interval is not identifying every causal gene. [ref]
The Genetics of Speciation by Reinforcement by Daniel Ortiz-Barrientos and others. PLoS Biology 2, e416; crosses, mate discrimination and the genetic basis of enhanced isolation
This evidence makes an evolutionary response plausible and helps distinguish basal isolation from its subsequent enhancement.The most direct prospective test would use replicated experimental evolution. Start with the same partially isolated populations, allow contact in treatment lines, and vary the biological fitness consequences of hybrid offspring while retaining appropriately matched controls. Across generations, test discrimination in a common environment, measure actual hybrid production and follow parental and hybrid reproductive success. Lines must be independent experimental units. Artificially removing hybrids can demonstrate a possible response to selection, but complete elimination of all hybrid-mediated gene flow simplifies the problem that the natural hypothesis seeks to explain. Changes due to crowding, learning or laboratory adaptation must also be separated from inherited changes in mate discrimination. A field intervention changing encounter rates could be informative, but ethical and ecological constraints often make longitudinal natural contact zones preferable.
Finally, importance in speciation is a broader question than existence in one pair of species. Comparative data should estimate how often hybrid costs, geographical overlap and enhanced barriers coincide, controlling for divergence time, ecology and phylogenetic nonindependence. Ascertainment matters: conspicuous surviving hybrid zones may omit cases where contact caused fusion, exclusion or near-complete isolation. A stronger preference is evolutionarily consequential only if it reduces effective exchange or helps maintain distinct lineages. Its effect should be measured alongside habitat separation, seasonal timing and postzygotic isolation, because sequential barriers act on the individuals that reach each stage.
Convincing evidence combines hybrid costs, opportunity for contact, inherited enhancement of isolation and exclusion of competing selective explanations. reinforcement can complete or stabilize a separation already under way, but geographic differences in signals alone establish neither its mechanism nor its frequency as a cause of speciation.
Past exam of the zoology course of the University of Cambridge 2024 Paper ZM5 1 Solution by Codex 0 2026-10-20
Codex 0 2026-10-20behavioural plasticity can slow inherited change by buffering selection, or accelerate it by permitting persistence and exposing organisms to new selection. There is no general ranking without specifying the trait, environment and timescale. The immediate adjustment of an individual's animal behaviour is a change in expression. evolution of that response requires a change in inherited properties of a biological population. A learned innovation spreading through cultural inheritance is another form of transmitted change, which should be distinguished from a change in allele frequencies.
A reaction norm makes this distinction explicit. Suppose a behavioural measurement in environment is , with inherited variation in baseline and responsiveness . For illustration, let the favoured value be , and let relative genotype fitness be:The first term penalizes mismatch; the second represents a possible cost of responsiveness. This is a deliberately simple model, not a claim that all animal behaviour has one optimum. Its phenotypic selection gradient on baseline, holding fixed, is:Immediately after a change to , individuals with match the optimum and experience no mismatch selection on ; otherwise identical individuals with experience a gradient . Thus phenotypic buffering can reduce selection for inherited baseline change even when the response is highly beneficial. If , selection on responsiveness can nevertheless persist. Buffering one dimension of the phenotype does not stop all evolution.
This impeding effect is biologically plausible when animals can avoid adverse conditions. Moving to a cooler microhabitat can reduce exposure to heat and therefore weaken selection on heat tolerance. Switching food can similarly reduce selection on digestive performance for an avoided resource. These are conditional mechanisms: the relevant evidence would be reduced differences in survival or reproduction among inherited physiological variants, rather than mere observation that animals move or switch foods. learning can also allow several inherited variants to reach similar behavioural performance, weakening selection among them. Such buffering may preserve genetic variation, which can become consequential after later environmental change; slow immediate change can therefore coexist with greater long-term evolutionary potential.
Acceleration begins with the demographic problem. An inherited advantage cannot spread in a lineage that disappears before it is expressed or transmitted. A flexible response can allow individuals to survive and reproduce after an environmental shift, providing time for subsequent inherited adaptation and possibly evolutionary rescue. This need not increase the selection coefficient of a particular variant. Increasing the number of surviving individuals or generations available for selection can matter even while the per-generation gradient becomes smaller. A comparison of change per generation and total adaptation over a fixed number of years can consequently give different answers.
behavioural plasticity can also change which environments impose selection. A newly learned foraging technique may expose animals to a new resource, making inherited differences in handling, digestion or sensory discrimination important. habitat preference can alter encounters with competitors and mates; repeated use of a new host can influence gene flow when mating occurs there. The host fidelity of Rhagoletis pomonella provides evidence that host-associated actions can constitute a premating barrier. It demonstrates a route from animal behaviour to evolutionary consequences, but does not by itself establish that the initiating host shift was a plastic response. [ref]
Host fidelity is an effective premating barrier between sympatric races of the apple maggot fly by Jeffrey L. Feder and others. PNAS 91, pp. 7990–7994; three mark-and-recapture studies and host-associated gene flow
Establishing that historical sequence is necessary before counting the case as plasticity-led evolution.In the Baldwin effect, acquired adjustments change survival and the selection subsequently experienced by inherited variants. genetic accommodation can then refine the threshold, specificity or efficiency of an environmentally induced response. Its outcome may be greater phenotypic plasticity, a differently tuned response, or genetic assimilation, in which expression becomes less dependent on the original inducing condition. No step requires a learned action to be copied directly into DNA.
Experiments on spadefoot toad tadpoles provide relevant, though not exclusively behavioural, evidence. Populations that expressed the carnivore ecomorph more frequently showed refinement of associated resource-use performance and morphology under laboratory comparison. Such correspondence is predicted if recurrent induction exposes the expressed phenotype to selection. The comparison supports inherited refinement following environmental responsiveness, but contemporary populations are not a direct film of the ancestral transition, and their prior ecological histories could differ. [ref]
Plasticity-led evolution: evaluating the key prediction of frequency-dependent adaptation by Nicholas A. Levis and David W. Pfennig. laboratory competition and expression of the carnivore ecomorph in spadefoot toad tadpoles
Classic selection on heat-induced crossveinless wings in Drosophila melanogaster also showed that a previously induced phenotype could eventually appear without the inducing treatment. That is evidence for genetic assimilation, not direct evidence that behavioural innovations generally accelerate evolution. [ref]Genetic assimilation of an acquired character by Conrad Hal Waddington. Evolution 7, pp. 118–126; heat-induced crossveinless wings and selection across generations
The balance depends on cue reliability, environmental persistence and costs of phenotypic plasticity. A response based on a formerly reliable cue can become maladaptive after environmental change. A persistent new environment may favour a cheaper constitutive solution, whereas recurring variation can favour continued flexibility. Response delays, limited sensory discrimination and trade-offs between alternative activities can leave substantial residual selection. Conversely, sufficiently effective and inexpensive flexibility can remove much of the benefit of further inherited change. The availability of relevant genetic variation and its genetic covariance with other traits also constrain the response.
A decisive study would separate immediate adjustment from inherited divergence. Replicated populations could experience stable and fluctuating environments, with variation in access to a learned response or environmental cue. Descendants should then be assayed in a common garden experiment, both with and without that cue. Repeated measures estimate within-individual change; pedigrees or crosses estimate inherited reaction norm differences. Survival, reproduction, population persistence and changes in other traits must all be measured. Manipulating responsiveness requires controls for sensory damage, stress and general incapacity: disabling a neural process and then observing extinction would not isolate an evolutionary benefit of flexibility. Comparisons across species additionally require control for phylogenetic nonindependence and ecological opportunity.
The strongest conclusion is conditional: effective adjustment often weakens immediate selection on the buffered trait, while persistence, new ecological exposure and inherited refinement can increase cumulative evolutionary change. Those mechanisms can operate together within the same lineage; their relative importance is an empirical question rather than an intrinsic property of flexible animal behaviour.
There are unlisted articles, also show them or only show them.