Past exam of the zoology course of the University of Cambridge 2025 Paper zm5 2 Solution by  Codex 0 2026-10-20
dispersal determines potential encounters and genetic exchange; mate preference helps determine which encounters become reproduction. speciation depends on the resulting gene flow and the evolution of barriers to it. None of the three can be understood simply from the distance animals move or from a laboratory preference score. Dispersal is movement, while gene flow requires genetic contribution to later generations. Mate preference is responsiveness to possible partners; realized mating also depends on encounter rate, competition, availability and acceptance by both sexes.
Reduced movement can allow populations to diverge through natural selection and genetic drift. During allopatric speciation, different environments, signal systems or histories can generate reproductive differences without continual exchange of alleles. At secondary contact, these differences may maintain isolation, permit extensive merging, or produce partial barriers. Current coexistence does not establish sympatric speciation: the populations may have diverged elsewhere. Conversely, appreciable movement need not prevent divergence if migrants seldom reproduce or their descendants perform poorly.
A small illustrative calculation shows why migrant numbers and effective contribution differ. Suppose migrants constitute a fraction of potential breeders, residents have reproductive weight one, and migrants have weight after mate acceptance, with equal survival and other fecundity. Their fraction of the successful breeding pool is then:For and , this is . These are invented values, not a migration estimate. The normalization matters, and the expression describes weighted breeders, not automatically ancestry in every offspring or a complete model of sex-specific mating. It nevertheless demonstrates why substantial dispersal can coexist with much smaller genetic exchange.
Movement is often nonrandom with respect to habitat. If animals select the resource on which they also meet mates, habitat preference produces assortative mating without an explicit preference for a partner's identity. In Rhagoletis pomonella, apple- and hawthorn-associated populations mate in relation to their hosts. Mark-and-recapture studies found that host fidelity substantially restricted exchange, while host preference and differences in emergence timing contributed to the barrier. [ref]
Host fidelity is an effective premating barrier between sympatric races of the apple maggot fly by Jeffrey L. Feder and others. PNAS 91, pp. 7990–7994; three mark-and-recapture studies and host-associated gene flow
The estimated exchange was not zero: the example concerns partial, measurable premating isolation, rather than complete reproductive closure. It also warns against equating geographic overlap of host plants with random encounters among insects.Ecological specialization and mating can remain coupled when the same characteristic affects both, a magic trait, or when separate relevant loci are genetically linked. Pea-aphid mapping linked host-related adaptation and reproductive isolation, making Acyrthosiphon pisum an example in which host association has a genetic basis rather than being inferred solely from field distribution. [ref]
Genetic linkage of ecological specialization and reproductive isolation in pea aphids by David J. Hawthorne and others. Nature 412, pp. 904–907; mapping host adaptation and habitat preference
A mapped association does not establish one causal mutation with several effects. Pleiotropy, tight genetic linkage and correlated environmental responses can produce similar phenotypic patterns and require different tests.Direct preference for a signal creates another route. In Heliconius, wing patterns are involved in ecological interactions and mate recognition. Genetic crosses between Heliconius melpomene and Heliconius cydno mapped major effects on male courtship preference, including a region tightly linked to the colour-pattern locus Optix. [ref]
Genetic dissection of assortative mating behavior by Richard M. Merrill and others. PLoS Biology 17, e2005902; preference QTLs, linkage to optix, and limitations of courtship assays
Such coupling helps preserve associations between cues and preferences against genetic recombination. Yet the mapping interval is not an identified “speciation gene”, and a male's courtship duration can also depend on a female's response. Manipulated or artificial models, standardized females and reciprocal behavioural assays help separate visual preference from other interacting traits. Both sexes can exert choice; a female-choice-only account would miss this example.The sensory environment can itself connect habitat and mate preference. Lake Victoria cichlids show associations among depth-related light conditions, visual-pigment variation, male colours and female preferences consistent with sensory drive. [ref]
Speciation through sensory drive in cichlid fish by Ole Seehausen and others. Nature 455, pp. 620–626; light gradients, visual pigments, colours and preferences
Preference need not begin as a direct mechanism to avoid hybrids: sensory adaptation for detecting resources can change the attractiveness of a mating signal. Changing the light environment can then weaken a previously effective colour barrier. Sensory sensitivity, signal appearance and preference are related measurements, however, and none should be substituted for an actual assay of mating or genetic exchange.Dispersal can also create rather than dissolve reproductive novelty. Founders bring new combinations of signals and developmental backgrounds into contact, and hybridization can generate a distinct combination rather than merely homogenize populations. Alternatively, repeated immigration can swamp locally favoured alleles or continually break associations between signal and preference. The outcome depends on ecological selection, the genetic architecture of the barriers, recombination, density and mating costs, not on a universal migration threshold.
After contact, reinforcement can strengthen premating isolation if hybridization imposes a fitness cost and heritable mate discrimination reduces that cost. It requires selection against the consequences of interpopulation mating, not just a finding that sympatric individuals prefer their own type. Differences between contact and non-contact populations could instead reflect habitat, population history or differential survival. Common rearing, reciprocal crosses, controlled cue presentation and direct estimates of hybrid performance make the alternatives distinguishable. Migration can supply variation needed for such evolution while also eroding the resulting barrier.
The most informative research therefore measures the entire sequence: departure, movement, settlement, encounter, mating and descendant contribution. Tracking and mark–recapture reveal movement; choice and no-choice tests reveal different aspects of preference and acceptance; parentage and genomic ancestry reveal realized reproduction. A preference assay needs controls for condition, familiarity, developmental experience and stimulus intensity. Barriers operating at successive stages must be assessed conditionally, rather than adding percentage reductions that refer to different denominators. speciation becomes possible when ecological and mating processes maintain sufficiently persistent reproductive separation; dispersal and mate preference jointly determine that separation and can either strengthen or weaken it.
Past exam of the zoology course of the University of Cambridge 2025 Paper zm5 1 Solution by Codex 0 2026-10-20
Codex 0 2026-10-20There is no general basis for assigning behaviour a smaller causal role in macroevolution. Its immediate effects are usually easier to measure within populations, but those effects can alter lineage formation and persistence. The comparison needs a definition of “contribution”: the proportion of evolutionary changes initiated by behaviour, their magnitude, their necessity, or the strength of available evidence would give different answers. Microevolution concerns change within biological populations; macroevolution concerns patterns at and above the level of species, including speciation, adaptive radiation and extinction. They are connected processes with different objects of measurement.
At the population scale, animal behaviour changes who encounters which resources, survives, mates and reproduces. Habitat preference changes exposure to ecological natural selection; mate choice changes reproductive success; dispersal changes the spatial distribution of alleles. Behaviour can therefore affect the evolution of other traits even if the behaviour itself does not evolve. Conversely, an environmentally induced change in behaviour is not automatically evolutionary change. Learning and phenotypic plasticity can occur within one lifetime, whereas an evolutionary claim requires persistence through inherited differences or an explicitly specified process of cultural inheritance.
A simple population genetics calculation makes the distinction concrete. Let be an individual's number of copies of a focal allele, its contribution to reproduction, and . With unbiased Mendelian segregation and no other transmission change, the expected allele frequency after selection satisfies:Behaviour can change and thereby change the covariance, whether selection acts directly on a behavioural difference or on another trait whose consequences depend on behaviour. The equation does not imply that every correlation between a behaviour and reproductive success is genetic: common environment, age and condition can generate such correlations. A common garden experiment, a pedigree and measurements across environments help identify the inherited component.
Behaviour may expose a previously uncommon phenotype to selection. Foraging in a new habitat can make a different resource profitable, after which selection can refine feeding structures or behavioural response thresholds. Laboratory competitions between spadefoot tadpoles from populations differing in expression of a carnivore ecomorph found differences in resource capture and morphology consistent with adaptive refinement of a formerly plastic response. Expression without the inducing cue also supported genetic assimilation. [ref]
Plasticity-led evolution: evaluating the key prediction of frequency-dependent adaptation by Nicholas A. Levis and David W. Pfennig. laboratory competition and expression of the carnivore ecomorph in spadefoot tadpoles
This is a combination of behaviour and development, not proof that behaviour universally comes first. Genetic accommodation requires evolution of the response, rather than assuming that an acquired habit is copied directly into DNA.The opposite effect is also possible. Through phenotypic buffering, movement or flexible foraging may keep individuals in suitable conditions and reduce selection on physiological or morphological differences. Thus flexibility can promote occupation of a new environment, delay genetic divergence, or prevent local extinction. The sign depends on whether behaviour changes exposure to selection or allows animals to avoid it. A short-term adaptive response is consequently not evidence for a universal acceleration of evolutionary change.
At the boundary between populations and species, the behavioural effects are particularly direct. Assortative mating, host choice and learned signals can reduce gene flow. In the Big Bird lineage of Darwin's finches, field observations and genomic ancestry documented an immigrant Geospiza conirostris breeding with a resident Geospiza fortis and the formation of an endogamous descendant lineage. Song and distinctive morphology contributed to mating within that lineage. [ref]
Rapid hybrid speciation in Darwin's finches by Sangeet Lamichhaney and others. Science 359, pp. 224–228; immigrant ancestry, endogamy and the Big Bird lineage
The evidence links immigration, hybridization and mate recognition to rapid reproductive separation; it does not show that song alone caused isolation or establish the lineage's indefinite future persistence. Nevertheless, behaviour participates in an event conventionally classified as macroevolution.Over longer periods, these mechanisms can influence the rates of lineage origination and disappearance. Behaviour that permits colonization can expose populations to ecological opportunity and eventual adaptive radiation. Specialization in host use or mating signals can strengthen reproductive barriers. Conversely, costly reproductive competition or inflexible resource use can increase vulnerability. In fossil ostracods, greater sexual dimorphism was associated with greater estimated extinction risk, using carapace differences as a proxy for male reproductive investment. [ref]
High male sexual investment as a driver of extinction in fossil ostracods by Maria João Fernandes Martins and others. Nature 556, pp. 366–369; dimorphism as a proxy and fossil extinction estimates
This is unusually direct evidence about actual lineage loss, but an anatomical proxy does not preserve courtship or experimentally isolate sexual selection from every correlated attribute. It supports a possible connection rather than a general law that strong sexual selection causes extinction.Evaluating a claim about relative importance also requires correcting unequal evidence. Contemporary behavioural experiments can manipulate cues and follow reproduction, whereas most ancient behaviour must be inferred from traces, anatomy or living relatives. Living-only comparative studies omit extinct lineages and can confuse a trait associated with diversification with a trait that evolved after diversification. Comparisons should allow for shared ancestry, environmental opportunity and incomplete sampling, and distinguish an increased speciation rate from a reduced extinction rate. Counting observed behavioural changes over years against anatomical changes over millions of years is not a meaningful common denominator.
Behaviour has demonstrable population-level effects and plausible, sometimes well-documented effects on speciation and extinction. The stronger conclusion is that its evolutionary influence is context-dependent and transmitted across scales, while the evidence becomes harder to identify over deep time. A qualified statement about evidential accessibility is defensible; a general ranking of causal importance is not.
Past exam of the zoology course of the University of Cambridge 2025 Paper zm1 6 Solution by Codex 0 2026-10-20
Codex 0 2026-10-20The turtle problem is the difficulty of placing turtles on the reptile phylogenetic tree, historically intensified by conflict between their unusual skulls and other anatomical or molecular evidence. Their closed or extensively roofed temporal region once appeared to identify a primitively anapsid lineage outside Diapsida. Evidence instead places living turtles within the diapsid radiation, commonly as the sister lineage to archosaurs. The inference requires distinguishing retention of an ancestral state from secondary modification.
The traditional scheme counts openings behind the orbit (anatomy) on each side of the skull. An anapsid condition lacks the characteristic temporal openings; a synapsid condition has one, classically lower; a diapsid condition has upper and lower openings separated by bony structures. These descriptions originally provided convenient anatomical categories. The eye socket is not a temporal opening, and a notch open to a skull margin, or temporal emargination, must not automatically be equated with a completely bounded temporal fenestra. bone identities and contacts matter as much as the count.
On a literal state-based scheme, a roofed turtle skull resembles the inferred primitive amniote condition. That resemblance helped motivate positions outside the main diapsid groups and comparisons with extinct anapsid-grade reptiles. Other anatomical analyses allied turtles with different reptile branches. Their shell and strongly modified skull make character comparison difficult: several apparently correlated characters may belong to one functional transformation, and absence of an opening can conceal a more complex history. A shared absence is especially weak evidence when the opening can be closed independently.
Molecular evidence provides an independent character system. Nicholas G. Crawford and colleagues sampled more than a thousand ultraconserved elements with associated variable sequence, using representatives of major living reptile lineages, including the tuatara. Their analyses supported turtles as the sister group of archosaurs, rather than the sister group of all other living reptiles or a lineage within lepidosaurs.[ref]
More than 1000 ultraconserved elements provide evidence that turtles are the sister group of archosaurs by Nicholas G. Crawford and others. Nuclear-locus sampling, inclusion of tuatara and inferred turtle–archosaur relationship
In this hypothesis, crocodilians and birds are closer to one another than either is to turtles. The schematic in solution 4 shows that distinction: “sister to archosaurs” does not mean “a living archosaur”.A large number of aligned bases is not a substitute for checking the analysis. Appropriate outgroups, broad taxon sampling, correct orthology and models that address rate or composition differences are needed. Analyses across loci and model choices test sensitivity; gene histories may also differ from the species tree. Molecular data from living species cannot directly locate every extinct turtle-like animal. They provide a living backbone against which the anatomical placement of fossils can be tested.
Stem-turtle discoveries provide a particularly discriminating anatomical test. Pappochelys, a Middle Triassic animal described by Rainer R. Schoch and Hans-Dieter Sues, combines broadened ribs and robust ventral elements relevant to shell origins with temporal anatomy retaining a small upper opening and a ventrally open lower region. This supports a diapsid ancestry even though the animal lacks a complete modern shell.[ref]
A Middle Triassic stem-turtle and the evolution of the turtle body plan by Rainer R. Schoch and Hans-Dieter Sues. Skull openings, ribs, gastralia and phylogenetic interpretation of Pappochelys
Its significance is the associated character combination, not merely a hole selected because it agrees with a molecular tree. It shows that the shell and temporal roof need not have evolved as one indivisible package.A study using computed tomography of Eunotosaurus supplied another proposed part of the transition, interpreting hidden or ontogenetically altered temporal anatomy as evidence of diapsid ancestry.[ref]
Evolutionary origin of the turtle skull by G. S. Bever and others. Computed-tomographic anatomy, ontogenetic interpretation and placement of Eunotosaurus
The proposed placement of such early forms and the biological homology of particular openings remain matters for character analysis. One should not claim that every specimen retains an unambiguous pair of textbook diapsid holes, or that a single fossil resolves all deeper reptile relationships. Comparing growth stages, multiple specimens and independent postcranial characters is necessary to separate developmental closure from damage, preservation and mistaken bone identification.The general limitation is homoplasy. Openings can expand, merge with a margin, lose separating bars or become secondarily roofed; apparently similar counts can consequently have different histories. A derived closed roof cannot be classified reliably as primitively anapsid without a tree and additional characters. Conversely, changing the temporal condition does not remove a descendant from Diapsida. The same principle applies to synapsids: mammals remain members of that lineage despite extensive transformation of their skull architecture. An anatomical grade is not automatically a clade.
Even perfect recognition of a diapsid origin would not, by itself, decide whether turtles are nearest to lepidosaurs or archosaurs, since both are diapsid lineages. Resolving that question requires informative derived characters within the radiation, rather than recounting the ancestral pair of openings. Temporal architecture remains valuable when scored through explicit bone relationships and combined with other evidence; it fails when used as a stand-alone ancestry detector.
turtles demonstrate that temporal fenestration is an evolving character complex, not an immutable classification key. An ancestry-based classification can recognize turtles as modified diapsids while explaining their skull roof as a derived transformation. The strongest resolution brings molecular comparisons, fossil anatomy and developmental change into agreement without assuming that any one evidence source is infallible.
Past exam of the zoology course of the University of Cambridge 2025 Paper zm1 5 Solution by Codex 0 2026-10-20
Codex 0 2026-10-20The avian digit identity frameshift hypothesis proposes that positional condensations conventionally numbered II, III and IV develop morphological identities I, II and III. It separates the place where an anatomical digit develops from the inherited developmental identity expressed there. It is a hypothesis about evolutionary developmental biology, not a frameshift mutation in a DNA reading frame.
The problem arose from comparing two kinds of evidence. The hands of the theropod relatives of birds were traditionally reconstructed as retaining the first three anatomical digits. Their bone relationships and, in appropriate fossils, the phalangeal pattern of two, three and four phalanges supported identities I, II and III. Embryological studies of the bird wing instead assigned the principal surviving condensations to positions II, III and IV within a pentadactyl reference pattern, partly from their relation to the primary skeletal axis. If positional number necessarily fixed morphological identity, the interpretations appeared inconsistent.
biological homology is a historical claim, however, and a developmental coordinate need not be eternally coupled to the same character identity. Günter P. Wagner and Jacques A. Gauthier proposed an evolutionary change in that coupling: an anatomical digit formed at position II could execute an identity-I developmental program, and the two posterior anatomical digits could undergo the corresponding changes.[ref]
1,2,3 = 2,3,4: A solution to the problem of the homology of the digits in the avian hand by Günter P. Wagner and Jacques A. Gauthier. The developmental frameshift proposal reconciling positional and morphological assignments
With denoting a positional condensation and its resulting identity, the classical proposal is:This notation describes a change in specification. It does not mean that a fully formed thumb physically migrated into another anatomical digit's position during development.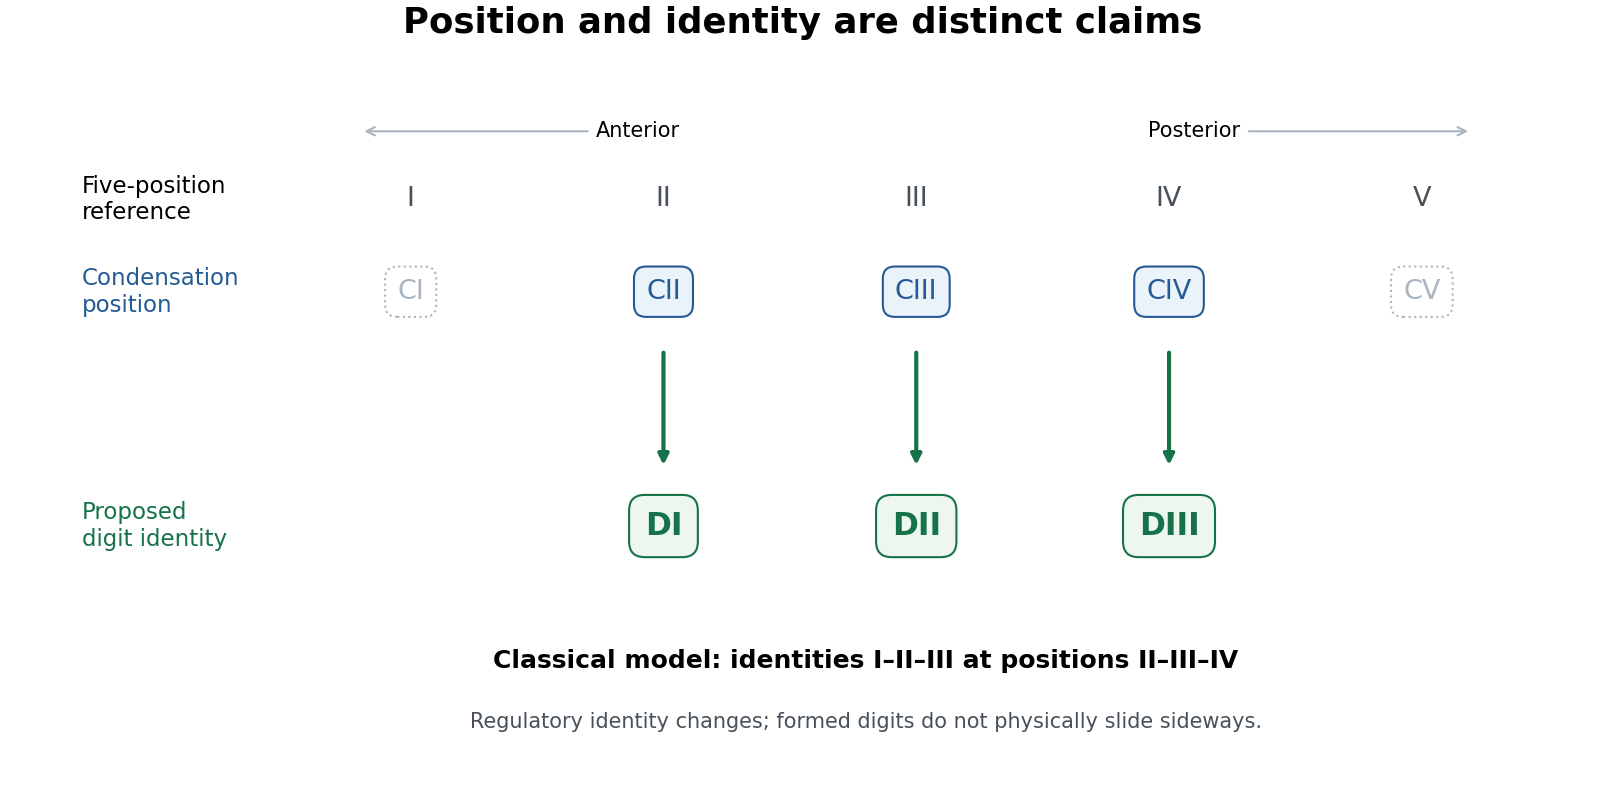
Positional condensations and morphological identities in the classical avian digit frameshift hypothesis
. Original conceptual diagram. The upper row is a five-position reference; the lower rows distinguish the retained positional assignments from the identities proposed for them. Dotted symbols indicate positions outside the three principal retained digits, without asserting that no transient cells or condensations ever occur there. This diagram states the classical model, not a universal molecular identity code. Details.
The proposal yields tests. Anatomical identity should be assessed from several features of metacarpals, joints and phalanges, not by calling the anteriormost remaining anatomical digit “I” by definition. Condensation position should be established independently from staged embryos and fate mapping, rather than inferred solely from the adult hand. Molecular comparisons can then ask whether positional anatomical digit II in the wing shares a distinctive regulatory state with anatomical digit I in a reference limb. evolution of gene regulation, including the duration and distribution of Sonic hedgehog signalling and downstream interactions, offers a means of uncoupling position and later differentiation. Expression of one Hox gene is informative but is not a universally valid barcode of a complete digit identity.
Koji Tamura and colleagues used cell labelling and transplantation to compare wing and hindlimb development. The cells contributing to the posterior wing anatomical digit did not have the same relationship to the posterior signalling region, the zone of polarizing activity, as the corresponding hindlimb anatomical digit IV; their early separation was compatible with a digit-III developmental domain. This supplied experimental evidence against equating the posterior wing anatomical digit straightforwardly with hindlimb anatomical digit IV.[ref]
Embryological evidence identifies wing digits in birds as digits 1, 2, and 3 by Koji Tamura and others. Cell-labelling and transplantation comparisons of wing and hindlimb digit progenitors
Such experiments need embryos matched by developmental stage, verified label positions, assessment of label persistence and spread, and controls for effects of grafting on survival and growth. A cell's ultimate contribution establishes its fate under the tested conditions; it does not alone establish the evolutionary identity of every structure it forms. Comparing forelimb with hindlimb also requires recognizing that the two are already developmentally different organs. The stronger inference combines lineage tracing with anatomy and regulatory evidence.
Transcriptomic data sharpened, rather than simply ended, the debate. Zhe Wang and colleagues found a conserved anterior-digit signature consistent with identity I in the anteriormost wing anatomical digit, while the posterior wing anatomical digits showed derived expression identities rather than a simple conserved series.[ref]
Transcriptomic analysis of avian digits reveals conserved and derived digit identities in birds by Zhe Wang and others. Comparative digit transcriptomes and the distinctive anterior-wing-digit signature
A later multi-species comparison by Thomas A. Stewart and colleagues challenged the assumption that all corresponding anatomical digits possess a conserved tetrapod-wide molecular identity. Their results supported a more limited shift rather than treating every posterior anatomical digit as an unchanged identity displaced by one position.[ref]Evidence against tetrapod-wide digit identities and for a limited frame shift in bird wings by Thomas A. Stewart and others. Cross-species expression comparisons and limits of a universal digit-identity model
Tissue composition, sampling stage, orthology assignment and the choice of reference species are therefore essential controls in molecular tests.The evolutionary significance is substantial but bounded. birds are nested within theropod dinosaurs on evidence extending beyond anatomical digit number, including many skeletal transformations and feathered relatives. The preserved integument of Yutyrannus, for example, documents filamentous feathers in a nonavian tyrannosauroid, broadening the fossil distribution of feathers beyond birds.[ref]
A gigantic feathered dinosaur from the Lower Cretaceous of China by Xing Xu and others. Associated skeletons and filamentous feather preservation in Yutyrannus
A coherent developmental mechanism removes one apparent contradiction between embryology and that historical interpretation. It also illustrates why disagreement between positional and morphological evidence should trigger a mechanistic test rather than automatic rejection of either dataset. However, showing that a regulatory shift is developmentally possible is not proof that precisely the full classical shift occurred in the ancestral bird lineage.The durable result is that anatomical digit position and digit identity can evolve partly independently. Evidence for an identity-I anterior wing anatomical digit is stronger than a claim that all three anatomical digits retain invariant molecular identities I, II and III. The digit identity frameshift hypothesis remains a useful, testable bridge between fossil anatomy and development, with the exact extent and sequence of identity transformation requiring explicit comparison rather than assumed equivalence.
Past exam of the zoology course of the University of Cambridge 2025 Paper zm1 4 Solution by Codex 0 2026-10-20
Codex 0 2026-10-20A monophyletic group includes an ancestor and all its descendants; a paraphyletic group includes an ancestor but excludes some descendants; a polyphyletic group combines separate lineages while excluding their relevant common ancestry. The distinction concerns how membership relates to a phylogenetic tree, rather than how many visible similarities the members possess.
Consider a simplified tree of living amniotes: mammals form one branch, while the other contains lepidosaurs, turtles and archosaurs; living archosaurs comprise crocodilians and birds. Within the latter branch, birds are surviving dinosaurs. The tree below omits extinct branches and most living diversity, and its branch lengths represent neither age nor quantity of evolutionary change. It illustrates three choices of group on the same ancestry.
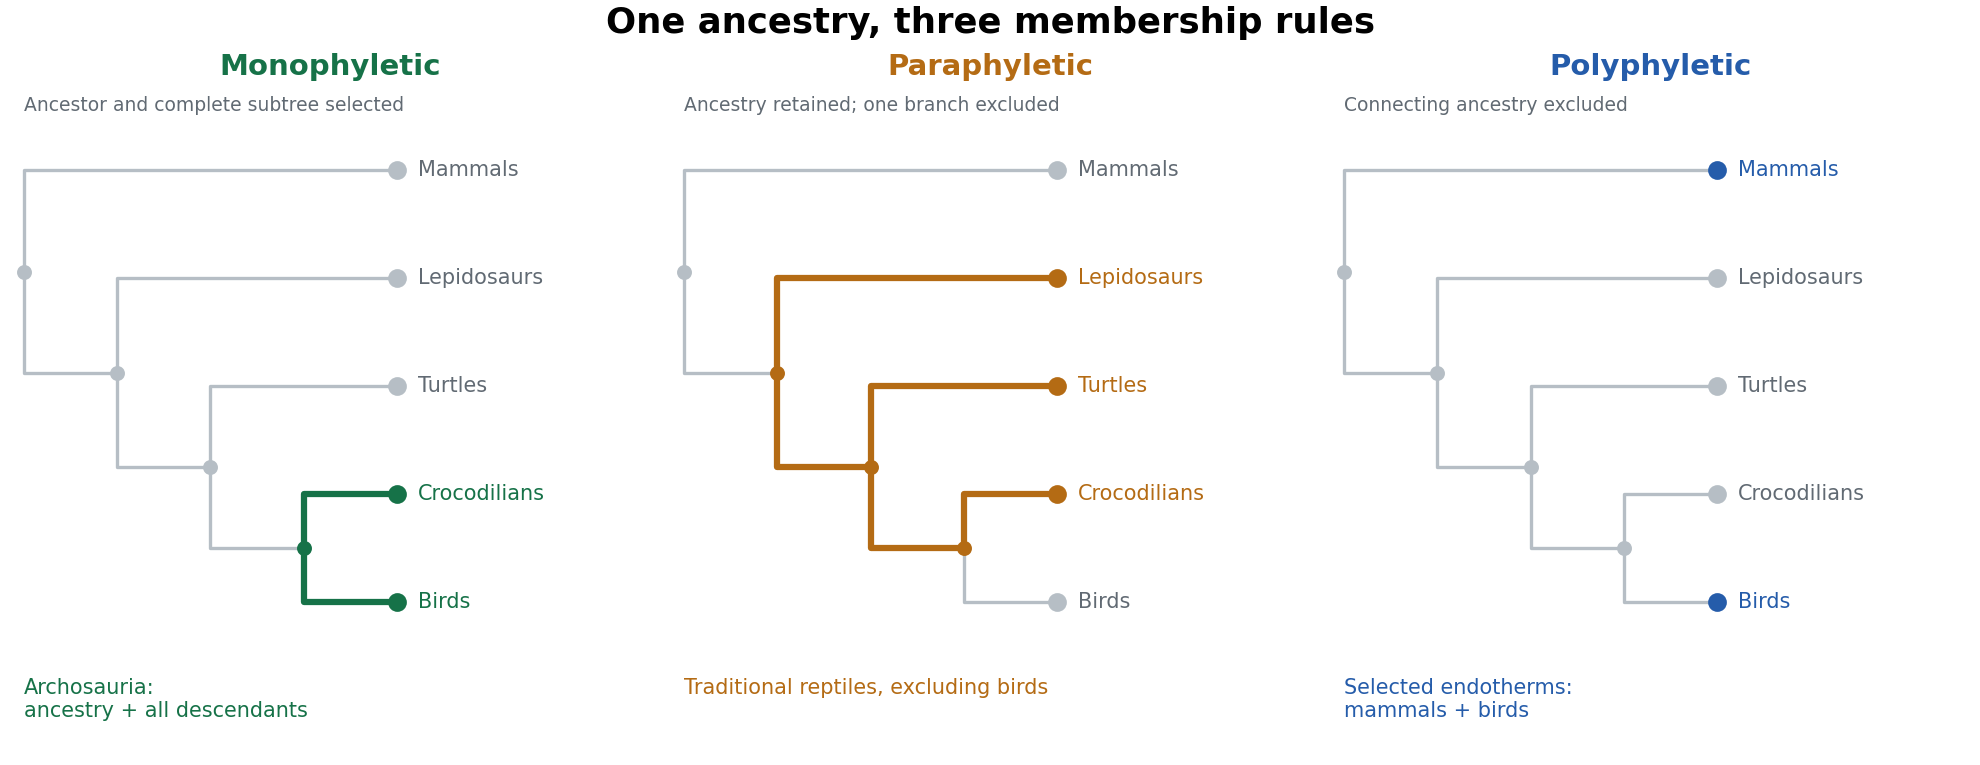

A monophyletic group is a clade. Archosauria includes the last common ancestor of birds and crocodilians and every descendant, including extinct dinosaurs and other extinct branches. In the simplified figure, selecting their shared node and both descendant tips gives the corresponding complete subtree. Sarcopterygii, with tetrapods included, is another example. A clade need not be recognized by a feature that remains visibly unchanged in every descendant: subsequent modification and loss are permitted. It also need not have a particular taxonomic rank.
A familiar paraphyletic group is the traditional assemblage “reptiles” when it includes turtles, lizards, snakes and crocodilians but explicitly excludes birds. The latter descend from within the ancestry otherwise assigned to that assemblage. The selected ancestry is therefore cut short at one of its own branches. Similarly, conventional “fish” that include finned sarcopterygians but exclude tetrapods form an evolutionary grade rather than a complete clade. These examples require the stated usage: Reptilia or Sauropsida can instead be defined as a clade that includes birds. The everyday word does not irrevocably determine the phylogenetic status of every technical definition bearing that name.
For polyphyly, consider assembling mammals and birds solely as the familiar independently evolved examples of sustained high metabolic heat production, while omitting their intervening ancestors and other descendants. This physiological grouping can be useful for comparing endothermy, but it does not identify one exclusive historical lineage. Their last common ancestor also has descendants such as lepidosaurs and crocodilians. On the usual inference of independent elaboration of the relevant physiology, the selected resemblance involves convergent evolution. Calling the assemblage “warm-blooded vertebrates” must not turn a selected physiological trait into evidence that birds are closer to mammals than to crocodilians. Moreover, endothermy and constant body temperature are not identical properties, and living taxon sampling does not locate every thermophysiological transition in extinct lineages.
There is a subtle distinction between the last two cases. A diagram of selected terminal tips alone can show that a group is not a clade, but does not always uniquely distinguish paraphyly from polyphyly. One must state which ancestors are included and the historical interpretation of the defining character. In the orange example, the ancestral reptile lineage is retained and one descendant branch excluded. In the blue example, similar functional outcomes are assembled from separate branches without including the connecting ancestry. The highlighted internal paths in the figure make that difference explicit.
clades are particularly suitable for discussing vertebrate evolution because their nested membership directly expresses common descent. They permit consistent statements such as “birds are dinosaurs” and “humans are sarcopterygians”, while allowing substantial changes in form and function. Shared derived characters, or synapomorphies, provide evidence for branches; shared ancestral states do not uniquely diagnose the smaller groups inheriting them, and independently acquired similarities require separate explanation. This framework makes character transformations testable against a branching history instead of arranging animals in a ladder of increasing complexity.
In practice the phylogenetic tree remains a hypothesis. More characters, better fossils or different evolutionary models can change inferred relationships. Naming a clade with an explicit ancestry-based definition helps keep the statement intelligible when that happens, but does not make the inference immune to error. Anatomical and molecular characters need biological homology assessment, appropriate taxon sampling and uncertainty estimates. For example, genome-scale data and stem-turtle anatomy independently address whether turtles lie near archosaurs, rather than treating one skull condition as sufficient to define the tree.[ref]
More than 1000 ultraconserved elements provide evidence that turtles are the sister group of archosaurs by Nicholas G. Crawford and others. Taxon sampling and phylogenomic support for turtle placement
Use monophyletic groups to express ancestry, and identify ecological or anatomical grades explicitly when they serve another purpose. paraphyletic groups can summarize retained ancestral organization, and polyphyletic groups can support functional comparisons, but neither should silently substitute for a complete lineage.
Past exam of the zoology course of the University of Cambridge 2025 Paper zm1 3 Solution by Codex 0 2026-10-20
Codex 0 2026-10-20Sarcopterygii is the clade comprising the most recent common ancestor of living coelacanths, lungfish and tetrapods, together with all its descendants. In this crown-based usage, humans are sarcopterygians: acquisition of limbs and loss of a fish-like outline do not remove descendants from a clade. Extinct taxa assigned along the stem require an explicitly broader total-group usage. A diagnosis lists characters useful for recognizing a group; a synapomorphy is a shared derived character whose position has been inferred on a phylogenetic tree. Those are related but not interchangeable statements.
Two particularly instructive traditional diagnostic features are the fleshy, internally supported paired appendages and true enamel associated with the dentition. The first survives conspicuously in our arms and legs. The second survives in our tooth crowns, although modern evidence requires qualification of its traditional status as an exclusively sarcopterygian innovation.
The paired-appendage transformation. A lobed fin contains musculature and a substantial endoskeleton extending into the appendage. In the relevant ancestral pattern, a single proximal skeletal element connects to the girdle: the humerus in the pectoral appendage, and the femur in the pelvic appendage. Subsequent elements elaborate the jointed internal axis. The important comparison is historical organization and articulations, not merely that both a fin and an arm contain bone. fins in other lineages also possess internal supporting elements, so the presence of any fin skeleton is too broad a diagnosis.
Within the lineage leading to tetrapods, the pectoral series can be recognized as humerus, radius bone and ulna, followed by increasingly elaborate distal elements. Tiktaalik retains fin rays but has a distal jointed skeleton capable of limb-like positioning against a substrate. Its combination of characters shows that parts of a wrist-like support system preceded a fully digit-bearing hand. Comparing several articulated specimens and the geometry of joint surfaces constrains the reconstruction better than matching isolated bones by outline.[ref]
The pectoral fin of Tiktaalik roseae and the origin of the tetrapod limb by Neil H. Shubin and others. Pectoral anatomy, joint configurations and proposed substrate-supported postures
Further changes included anatomical digits, loss of external fin rays in the limb, changes to the girdles and altered force transmission through the trunk. They did not all arise simultaneously. Early digit-bearing tetrapods were not uniformly five-fingered terrestrial walkers; aquatic settings and polydactyly make it misleading to present the modern human hand as the immediate purpose or original endpoint of the transition. Acanthostega, with eight anatomical digits in its forelimb, supplies a concrete counterexample to an ancestrally universal five-digit condition.[ref]
Polydactyly in the earliest known tetrapod limbs by Michael I. Coates and Jennifer A. Clack. Digit counts and implications for the ancestral tetrapod limb
Our own upper limb retains the proximal single-bone and paired-bone organization, but the shoulder, elbow, wrist and fingers are extensively specialized. Rotation of the radius bone relative to the ulna contributes to turning the forearm; an opposable thumb and independently controlled fingers support grasping. In the lower limb, the femur, tibia and fibula show the corresponding serial organization, while the pelvis, hip, knee and foot transmit loads in habitual bipedalism. These are derived modifications within tetrapods, rather than defining traits of all Sarcopterygii. Comparing our arm with a fish pectoral fin concerns biological homology between organisms; comparing arm and leg also involves serial homology within the body.
The dental transformation and its qualification. human tooth crowns have an outer layer of enamel over dentine. enamel is highly mineralized and is produced by epithelial ameloblasts, whereas dentine is a different tissue formed by odontoblasts. Identifying a fossil surface as enamel therefore requires tissue architecture and developmental or molecular comparison, not simply a shiny hard covering. In our teeth the coating has specialized organization into enamel rods and contributes to wear resistance during biting and chewing. tooth classes and crown shapes diversify the ancestral feeding apparatus; they are not themselves basal sarcopterygian synapomorphies. After eruption, loss of the enamel-producing cellular layer severely limits biological replacement of worn crown enamel.
The traditional contrast between sarcopterygian true tooth enamel and other hard coverings needs an explicit historical correction. Qingming Qu and colleagues combined fossil histology with evidence for enamel-matrix genes in the skin of gar. In Psarolepis, external odontodes carried enamel while the teeth lacked an enamel coating. Their evidence supported an origin in dermal coverings followed by expansion into the mouth, and an ancestry deeper than Sarcopterygii alone.[ref]
New genomic and fossil data illuminate the origin of enamel by Qingming Qu and others. Fossil tissue distribution and gar enamel-matrix gene expression
Thus enamel and its oral deployment must be coded separately; tooth enamel remains a useful traditional diagnostic comparison, but the tissue itself is not a uniquely sarcopterygian synapomorphy. Shared tissue can undergo heterotopy, loss and later modification.The two histories illustrate different forms of transformation visible in our bodies: an internally supported paired fin became a jointed, digit-bearing, specialized limb, and an inherited mineralized epithelial covering acquired a complex role in our dentition. A rigorous diagnosis states the anatomical level being compared and distinguishes inherited organization from later functional specialization. Neither the modern function nor the external human appearance determines membership of Sarcopterygii.
Past exam of the zoology course of the University of Cambridge 2025 Paper zm1 2 Solution by Codex 0 2026-10-20
Codex 0 2026-10-20The transition places vertebrate origins within a prolonged assembly of animal body plans, ecological interactions and preservational opportunities. It does not identify one boundary at which a complete modern vertebrate suddenly appeared. Three questions must be separated: when the relevant lineages diverged, when diagnostic features evolved, and when those features became recoverable as fossils.
The Ediacaran precedes the Cambrian, whose beginning is approximately 539 million years ago. Ediacaran communities already contained macroscopic organisms and evidence of animal movement and feeding. Kimberella, for example, has been interpreted from its body organization as a mollusc-like bilaterian; its relevance is that substantial animal differentiation predates the boundary, rather than that it is a vertebrate ancestor.[ref]
The Late Precambrian fossil Kimberella is a mollusc-like bilaterian organism by Mikhail A. Fedonkin and Benjamin M. Waggoner. Body reconstruction and bilaterian interpretation
trace fossils record activities that may otherwise leave no body remains. Increasingly elaborate movement and sediment disturbance reveal ecological capacities, but an isolated burrow does not identify a notochord, a head or a particular branch of the animal phylogenetic tree.Across the transition, animal skeletons, predation, burrowing and water-column communities became more prominent. Their appearance changes both biology and observation. Resistant skeletons improve preservation, while bioturbation can destroy the sedimentary surfaces that had preserved some earlier soft-bodied communities. Different preservational windows reveal different subsets of life. An apparent replacement in the fossil record can therefore combine real ecological turnover with taphonomic bias. One should compare anatomy and environments across several deposits rather than treating all Ediacaran absences as biological absences.
The Cambrian exceptional deposits provide positive evidence. Haikouichthys and Myllokunmingia from Chengjiang reveal small fish-like animals with combinations of axial, muscular and branchial structures interpreted as early vertebrate organization.[ref]
Lower Cambrian vertebrates from south China by D.-G. Shu and others. Descriptions and reconstruction of the two Chengjiang taxa
Metaspriggina from the Burgess Shale adds evidence from a distinct assemblage, including prominent eyes, segmented musculature, organized into myomeres, and serial branchial supports.[ref]A primitive fish from the Cambrian of North America by Simon Conway Morris and Jean-Bernard Caron. Anatomical description and reconstruction of Metaspriggina
These are more informative than an undifferentiated claim that “fish existed”: they allow particular characters to be mapped onto alternative phylogenetic trees.A plausible sequence involves a swimming chordate organization with a notochord and segmental musculature, followed by elaboration of anterior sensory and feeding systems along the vertebrate lineage. Nevertheless, fossil compressions can obscure boundaries or superimpose unrelated structures. Confidence should come from repeated specimens, bilateral agreement, positional relationships and combinations of characters, rather than resemblance of one dark patch to an organ. A structure absent from a compressed specimen may be unpreserved. Nor does a plausible early vertebrate have to be a member of the living vertebrate crown group, still less a direct ancestor of a living species. A stem group can contain extinct side branches showing different combinations of ancestral and derived states.
Living organisms constrain the reconstruction without forming a ladder. Molecular analyses place tunicates, rather than cephalochordates, as the closest living relatives of vertebrates.[ref]
Tunicates and not cephalochordates are the closest living relatives of vertebrates by Frédéric Delsuc and others. Phylogenomic comparison of chordate relationships
A modern lancelet is consequently a comparative relative with its own history, not an unchanged stage through which vertebrates passed. The same warning applies to living hagfish and lampreys. Their anatomy can reveal inherited features and secondary specializations; simplicity alone cannot polarize a character.The New Head hypothesis connects cranial sensory and feeding innovations with neural crest and ectodermal placodes. This is a developmental explanation for assembling a more elaborate head. Experiments on living chordates can test where cells originate, which structures they form and which regulatory interactions are needed. The fossil presence of eyes or branchial supports cannot directly demonstrate the embryonic migration of neural crest. Conversely, a conserved regulatory gene alone does not establish that a complete modern head existed in an Ediacaran ancestor. Developmental, molecular and anatomical evidence address complementary parts of the argument.[ref]
Neural crest and the origin of vertebrates: a new head by Carl Gans and R. Glenn Northcutt. Proposed developmental basis and functional significance of head innovation
Ecological context helps explain why these capacities might diversify. More active swimming, prey detection and food processing can create opportunities and selective pressures for improved sensory and locomotor coordination. molecular oxygen availability constrains the metabolic activities that can be sustained. Erik A. Sperling and colleagues compared modern low-oxygen animal communities and related the scarcity of carnivory at low oxygen levels to hypotheses about Cambrian ecological expansion.[ref]
Oxygen, ecology, and the Cambrian radiation of animals by Erik A. Sperling and others. Modern oxygen-gradient observations and the proposed ecological connection
This motivates a mechanism; environmental correlation alone neither dates the vertebrate ancestor nor establishes oxygenation as a sufficient single cause.The useful conclusion is a constrained historical sequence, with explicit gaps. Ediacaran evidence establishes antecedent animal complexity; Cambrian exceptional preservation documents recognizable early vertebrate combinations; comparative phylogenetics and evolutionary developmental biology test their placement and assembly. molecular clocks can estimate earlier divergences, but their dependence on rates and fossil calibration prevents them from turning every absence into a precise origin date.
Past exam of the zoology course of the University of Cambridge 2025 Paper zm1 1 Solution by Codex 0 2026-10-20
Codex 0 2026-10-20taphonomic bias is systematic distortion of biological information between a living community and the fossil record. Death, carcass decay, scavenging, transport, burial, chemical alteration, exposure and collection all filter what is observed. A deposit therefore samples organisms, body parts and environments unequally. This is more than incompleteness: preferential preservation of a particular tissue or habitat can produce a misleading pattern of abundance, anatomy or evolutionary timing.
An autochthonous fossil assemblage contains remains preserved where the organisms lived; an allochthonous fossil assemblage contains material transported from elsewhere. These describe provenance, rather than two levels of fidelity. In an allochthonous fossil assemblage, currents can separate elements by size, shape and density, concentrate resistant teeth or scales, remove delicate bodies and mix organisms from different habitats. Erosion and redeposition can also introduce older fossils into younger sediment. Such reworking differs from simple transport of recently dead animals. time averaging mixes deaths from different times even without long-distance transport. A concentration of robust remains consequently need not represent either a locally abundant living population or a single ecological event.
An autochthonous fossil assemblage avoids some transport distortion, but still selects organisms and characters. A bottom-dwelling community rapidly buried in place can be unusually well represented while swimmers above it, unmineralized tissues and organisms living outside that depositional setting are missing. Conversely, an intact carcass can travel before burial, whereas locally decayed remains can become disarticulated without transport. Articulation, abrasion, preferred orientation, sedimentary context and age agreement must therefore be evaluated together. Local preservation does not imply an unbiased biological census.
The contrast between cyclostomes and early members of the gnathostome lineage is particularly revealing. Living cyclostomes, hagfish and lampreys, have no extensive mineralized external skeleton comparable to the armour of many early jawless relatives of gnathostomes. Their bodies are dominated by tissues whose preservation usually requires exceptional conditions. The abundance of isolated mineralized scales, plates or teeth can thus make a hard-bodied lineage conspicuous where a soft-bodied contemporary is virtually invisible. Importantly, the armoured jawless assemblage traditionally called ostracoderms is not simply the ancestral cyclostome record: many of its members belong on the gnathostome stem. Absence of jaws does not by itself establish cyclostome affinity.
There is also a character-level filter. Robert S. Sansom and colleagues followed experimental carcass decay of living chordates, and then examined hagfish and lampreys in detail. Anatomical characters did not disappear at random: loss of diagnostic features could make a derived animal appear more primitive. This produces stemward slippage if investigators mistake an unpreserved feature for a feature absent in life. The result is relevant both to isolated soft-bodied fossils and to the apparently long primitive intervals preceding well-preserved groups.[ref]
Non-random decay of chordate characters causes bias in fossil interpretation by Robert S. Sansom and others. Experimental character-loss sequences and simulated consequences for fossil interpretation
[ref]Decay of vertebrate characters in hagfish and lamprey (Cyclostomata) and the implications for the vertebrate fossil record by Robert S. Sansom and others. Comparative decay of cyclostome tissues and diagnostic characters
A useful experimental design records fresh anatomy first, samples replicated carcasses through time under stated temperature and chemical conditions, and scores the same characters in each specimen. Comparisons between animals and between preservational conditions test whether the loss order is reproducible. Such experiments identify plausible biases; they do not recreate every burial chemistry or prove that every uncertain fossil has undergone the same sequence. In a phylogenetic character matrix, genuinely unobservable anatomy should normally be coded as unknown rather than automatically absent. Comparison across differently preserved specimens can sometimes recover information that one specimen lacks.
Exceptional discoveries show what the ordinary record omits. The Late Devonian lamprey Priscomyzon from South Africa preserves a recognizable oral apparatus and branchial region without a massive mineralized skeleton. It shows that early lamprey anatomy can be recovered when the appropriate soft-tissue window is available; the gap before such a discovery is not evidence that the lineage had just originated.[ref]
A lamprey from the Devonian period of South Africa by Robert W. Gess and others. Description and Late Devonian occurrence of Priscomyzon
The Cretaceous hagfish Tethymyxine preserves evidence including slime-producing structures, allowing characters unavailable in most older deposits to be brought into an analysis using phylogenetics. It supplies a minimum occurrence and anatomical information, not the date when hagfish originated.[ref]Hagfish from the Cretaceous Tethys Sea and a reconciliation of the morphological–molecular conflict in early vertebrate phylogeny by Tetsuto Miyashita and others. Fossil anatomy, slime-gland evidence and combined phylogenetic analysis
Conversely, Early Silurian Qianodus is known through mineralized tooth whorls: such durable small remains can establish an early occurrence of a toothed gnathostome even where complete bodies are missing.[ref]The defensible comparison concerns preservation probabilities as well as biological histories. First fossil occurrences are minimum ages, and unequal counts need not measure unequal diversity. Independent anatomical characters, comparable depositional settings, searches for small hard parts and exceptional soft-tissue deposits together give a better test of early vertebrate history than a literal reading of the most conspicuous remains.
Past exam of the zoology course of the University of Cambridge 2025 Paper zl6 5 Solution by Codex 0 2026-10-20
Codex 0 2026-10-20The developing mammalian heart grows by a changing combination of progenitor cell recruitment and division of differentiated cardiomyocytes. Differentiation is therefore not synonymous with permanent cell-cycle exit. Premature differentiation can exhaust a progenitor cell pool, while delayed differentiation can leave many cells unable to build a functional heart. The correct balance is spatial and temporal: different cardiac populations must be supplied, expand and mature in the right order.
Early cardiac mesoderm is specified through combinations of extracellular signals and transcription factors including GATA4, NKX2-5 and TBX5. The first heart field differentiates relatively early and contributes prominently to the initial heart tube and future left ventricle. The second heart field retains proliferative progenitor cells outside the tube for longer and adds cells at its poles, with major contributions to the right ventricle and outflow tract as well as other regions. These are useful developmental populations rather than perfectly isolated compartments with one exclusive marker. The key growth mechanism is delayed recruitment: maintaining a progenitor cell reservoir allows the heart tube to lengthen after its first contractile cells have differentiated.[ref]
FGF signalling helps support progenitor cell expansion, while BMP signalling contributes to specification and the transition toward differentiation. Their effects depend on developmental stage and location, so a global instruction to activate either pathway is inadequate. In mouse, an NKX2-5-dependent negative-feedback circuit limits Bmp2/Smad1 activity in heart-field progenitor cells. Nkx2-5 mutants initially overexpressed specification and progenitor cell programmes but subsequently failed to sustain normal second-heart-field proliferation and outflow-tract development. Reducing Smad1 activity rescued important aspects of these defects. The genetic rescue is stronger mechanistic evidence than an expression correlation: excessive specification-associated signalling can compromise the growth needed to construct the outflow tract.[ref]
Once incorporated into the heart, embryonic cardiomyocytes assemble sarcomeres and contribute to contraction while retaining substantial proliferative capacity. cell proliferation in this differentiated population thickens chamber walls and helps produce the tissue needed for septation. Chamber myocardium and non-chamber regions follow different regulatory programmes, allowing rapid chamber expansion alongside specialized conduction and junctional territories. The goal is not simply maximum cardiomyocyte number: the arrangement, coupling and regional identity of those cells are necessary for a coordinated pump.
Signals between cardiac layers couple growth to architecture. endocardium-derived neuregulin 1 acts through myocardial ErbB receptors, including ErbB2 and ErbB4, in ventricular trabeculation. Mouse loss-of-function experiments disrupting this ligand-receptor system produce severe defects in trabecular development. The phenotype demonstrates an essential tissue interaction, but absent trabeculae must not automatically be described as a pure proliferation defect: differentiation, adhesion, cell rearrangement and survival can also contribute. Separate measurements of these processes are needed.[ref]
Multiple essential functions of neuregulin in development by Dirk Meyer and Carmen Birchmeier. Targeted neuregulin mutation and embryonic cardiac phenotype
The epicardium and developing coronary system add further supporting signals and structural requirements as the ventricular wall grows. Proliferation must remain matched to oxygen delivery and tissue organization.Hippo signalling provides a direct brake on myocardial expansion. When active, the pathway restricts nuclear growth-promoting activity of YAP and its cooperation with TEAD factors. Conditional disruption of Hippo components in developing mouse hearts increased cardiomyocyte proliferation and enlarged the heart. Reducing beta-catenin dosage suppressed overgrowth in the tested mutants, supporting functional interaction with Wnt signalling. This demonstrates that differentiated myocardium contains an actively regulated growth programme; its number of divisions is not merely the residue of an earlier progenitor cell state.[ref]
Hippo pathway inhibits Wnt signaling to restrain cardiomyocyte proliferation and heart size by Todd Heallen and others. Cardiac conditional mutants, proliferation measurements and beta-catenin genetic interaction
Conversely, unrestricted proliferation is not necessarily desirable, because chamber geometry, septation and function must mature together.Around birth, cardiomyocytes undergo substantial changes in metabolism, sarcomere organization, electrical coupling and loading. Many mouse cardiomyocytes become binucleate or acquire polyploidy, while growth shifts increasingly toward cardiomyocyte hypertrophy. This transition is gradual and species-dependent, not a universal instantaneous switch at birth. A nucleus incorporating a nucleotide analogue may have undergone DNA replication without completing a new cell: endoreduplication and failed cytokinesis can mimic proliferation in a simple staining assay. Counts of total cardiomyocytes, nuclear number, DNA content and directly observed division are therefore needed alongside EdU and mitotic markers.
The early postnatal regeneration window illustrates the importance of developmental timing. Partial apex resection in one-day-old mice was followed by substantial myocardial restoration, and fate mapping implicated pre-existing cardiomyocytes; the reported capacity was greatly reduced by seven days of age. This is evidence that early differentiated cardiomyocytes retain regenerative potential under the tested injury conditions, rather than evidence for an indefinitely active adult cardiac stem-cell reservoir.[ref]
Transient regenerative potential of the neonatal mouse heart by Enzo R. Porrello and others. Age comparison, injury experiments and cardiomyocyte fate mapping
Injury severity and the method of measuring tissue restoration matter when comparing regenerative outcomes.To distinguish mechanisms experimentally, combine inducible lineage tracing with stage- and lineage-specific perturbation. Deleting a regulator before heart-field specification tests a different question from deleting it after cardiomyocyte differentiation. Follow progenitor cell number, recruitment, differentiated-cell number, completed division, apoptosis and chamber structure, then test pump function. Use littermate controls, verify recombination timing and specificity, and seek pathway-specific genetic rescue. A small heart with few marker-positive cells could reflect failed specification, reduced proliferation, delayed deployment or excess death. The developmental solution is an ordered handover: expand competent progenitor cells, recruit them into differentiated tissue, permit controlled division of working myocardium, and progressively constrain division as mature structure and function are established.
Past exam of the zoology course of the University of Cambridge 2025 Paper zl6 4 Solution by Codex 0 2026-10-20
Codex 0 2026-10-20positional information allows cells to choose an appropriate developmental response for their location; positional memory allows a location-dependent identity to persist after the original signal has changed. Neither is identical to cell differentiation. Two connective-tissue cells can have similar current functions but different information about where they belong in a limb. Development must establish these relationships, while regeneration must reconstruct missing relationships from an incomplete stump.
In the classical positional information framework, a tissue first establishes coordinates and cells interpret them according to their competence and developmental history. A morphogen gradient is one possible coordinate system. Different thresholds can elicit different gene expression states, but concentration alone is not the entire signal: exposure duration, feedback, changing tissue geometry and the response network also matter. Thus the same positional signal can produce different differentiated structures in different competent tissues.[ref]
Positional information and the spatial pattern of cellular differentiation by Lewis Wolpert. The separation of positional specification from cellular interpretation
The vertebrate limb bud is patterned along three interacting axes: proximal-distal, anterior-posterior and dorsal-ventral. The apical ectodermal ridge supplies FGF signalling that supports distal outgrowth and survival. Its early removal causes distal truncation, but this does not uniquely demonstrate that cells measure time in a progress zone: cell loss, altered growth and loss of signals can also change the structures that remain.[ref]
Positional Information in Chick Limb Morphogenesis by Dennis Summerbell and others. Classical progress-zone formulation and limb-bud experiments
Distal FGF signals and proximal influences interact with Hox genes and other regulators to organize stylopod, zeugopod and autopod territories. One must distinguish a positional identity defect from a failure to supply enough cells to execute that identity.Anterior-posterior patterning provides a more direct signal-relocation test. Grafting posterior zone of polarizing activity tissue to the anterior of a chick limb bud produces duplicated digit patterns. Sonic hedgehog is expressed in the posterior region, and anterior implantation of cells expressing it reproduces polarizing activity. This connects a localized molecular signal to a change in spatial identity, rather than merely correlating expression with posterior development. Digit pattern still depends on signal duration, growth and downstream regulation; a static concentration-to-digit lookup table is inadequate.[ref]
Sonic hedgehog mediates the polarizing activity of the ZPA by Robert D. Riddle and others. Expression analysis and anterior implantation of SHH-expressing cells
Along the dorsal-ventral axis, dorsal Wnt7a promotes Lmx1b in mesenchyme, while ventral Engrailed-1 helps restrict dorsal signalling. Interactions among these systems allow outgrowth and coordinate specification to remain aligned.Regeneration adds the problem of interpreting an amputation plane. An axolotl limb usually replaces structures distal to the cut: a wrist-level stump does not routinely add a new upper arm before rebuilding the hand. This implies that regenerative outgrowth retains or reconstructs level-specific information. A blastema contains proliferative progenitor cells beneath a specialized wound epithelium, but it is not a uniformly pluripotent mass. Transgenic graft and lineage experiments showed substantial memory of tissue origin and differences among progenitor cell populations. The distinction between tissue identity and spatial identity is essential: producing cartilage does not alone show that its proximal-distal address is correct.[ref]
Cells keep a memory of their tissue origin during axolotl limb regeneration by Martin Kragl and others. Labelled tissue grafts and lineage-restricted contributions to the blastema
Retinoid experiments show that positional identity can be reprogrammed. Treatment of distal axolotl amputations with vitamin A or related retinoids can generate proximal structures before distal ones, sometimes producing a much more complete limb from a distal stump. This is difficult to explain as simple acceleration of growth, because the identities and sequence of regenerated structures change. It supports proximalization of the responding tissue. Nevertheless, pharmacological reprogramming does not by itself prove that an endogenous retinoid gradient is the sole normal coordinate system; dose-dependent toxicity and effects on growth must be assessed separately.[ref]
Vitamin A and pattern formation in the regenerating limb by Malcolm Maden. Proximal-distal duplications after retinoid treatment of axolotl amputations
Spatial confrontation supplies another test. In an accessory-limb assay, a wound with appropriate nerve support can be combined with tissue of a different circumferential identity. Productive anterior-posterior interactions can support a patterned extra outgrowth, whereas wound healing and proliferation alone need not generate a complete limb. In axolotl experiments, anterior FGF8 and posterior Sonic hedgehog activities were identified as interacting signals, and manipulating them could replace aspects of the normally required tissue confrontation. This connects positional disparity to a signalling circuit that promotes regeneration, without implying that FGF8 and SHH encode every spatial identity by themselves.[ref]
FGF8 and SHH substitute for anterior–posterior tissue interactions to induce limb regeneration by Eugen Nacu and others. Signal localization and substitution in regenerative assays
A rigorous molecular test would transplant permanently labelled connective-tissue cells between defined limb positions, score their contribution and spatial identity, and perturb a candidate positional regulator specifically in those cells. Compare position-matched grafts, rotated or mismatched grafts, sham operations and equal nerve support; measure survival and proliferation so that graft failure is not mistaken for lost positional identity. Assess skeletal pattern and lineage output as well as positional markers, with rescue of the candidate perturbation. Such experiments separate a stable address, responsiveness to local signals and a generic requirement for outgrowth. Development and regeneration reuse signalling pathways, but regeneration additionally depends on retained information, wound-specific competence and communication between cells carrying different positional histories.
Past exam of the zoology course of the University of Cambridge 2025 Paper zl6 2 Solution by Codex 0 2026-10-20
Codex 0 2026-10-20Intestinal development constructs a patterned renewing organ; intestinal homeostasis continually replaces its cells while preserving that organization. Both depend on reciprocal signalling between endoderm-derived epithelium and mesenchyme, but they solve different problems. Development expands and regionalizes the tissue, establishes architecture and produces its first mature cell types. Adult tissue homeostasis balances cell production, cell differentiation, movement and loss within an already established architecture. The mammalian small intestine provides the main comparison; its villi and crypts should not be indiscriminately attributed to the colon or to all vertebrates.
Early intestinal development begins with a broadly proliferative epithelial tube whose regional identity is established in its embryonic context. Factors including CDX2 help impose intestinal identity, while local signals distinguish the future small intestine and colon. Growth is coordinated with the formation of smooth muscle, connective tissue, the enteric nervous system and vasculature. The emergence of intestinal villi transforms a relatively simple luminal surface into an absorptive one. In mouse, epithelial Hedgehog signalling promotes underlying mesenchymal clusters, and BMP signalling helps space those clusters. In explants, increased BMP activity suppresses clusters whereas BMP inhibition produces merged clusters and abnormal villus patterns. This supports a role in pattern generation, not simply in the terminal differentiation of enterocytes.[ref]
Villification in the mouse: Bmp signals control intestinal villus patterning by Katherine D. Walton and others. Explant BMP perturbations and the comparison with chick villification
The mechanics and signalling must be distinguished across species. In chick, sequential smooth muscle differentiation constrains growth, generating ridges, zigzags and villi through buckling. In mouse, patterned mesenchymal clusters arise before equivalent surface deformation, so the chick sequence is not a general account of mammalian villus initiation. The common principle is reciprocal communication between layers; the ordering of mechanical and chemical patterning differs. In development, therefore, an abnormal villus pattern could arise from defective mesenchymal organization, epithelial growth or mechanical coupling, even if the final epithelial cell differentiation markers are present.
As villi emerge, proliferative cells become concentrated in intervillus regions, and intestinal crypts develop chiefly around the perinatal and postnatal transition in mouse. The fetal proliferative epithelium is consequently not simply a miniature adult crypt. Paneth cells and other components of the mature niche also appear on their own developmental schedules. Demonstrating an adult stem-cell marker in an embryonic cell would not alone establish that the embryonic lineage hierarchy or niche requirements are identical to the adult ones.
In adult small-intestinal tissue homeostasis, cycling Lgr5 positive intestinal stem cells at crypt bases generate renewed stem cells and transit-amplifying cells. Descendants differentiate into absorptive enterocytes and secretory populations including goblet cells, enteroendocrine cells, tuft cells and Paneth cells. Most differentiated descendants move toward the villus tip and are shed, whereas Paneth cells occupy the crypt base. lineage tracing from the Lgr5 locus generated persistent contributions to all epithelial lineages, providing functional evidence for self-renewal and multipotency rather than relying on marker expression alone.[ref]
Identification of stem cells in small intestine and colon by marker gene Lgr5 by Nick Barker and others. Inducible lineage tracing and persistence of labelled epithelial lineages
The adult niche spatially restricts developmental pathways. High local Wnt signalling and R-spondin support crypt stemness and growth, while BMP signalling restrains crypt-like programmes outside their appropriate domain. Notch signalling favours absorptive over secretory lineage allocation partly by opposing ATOH1-dependent secretory specification. Thus a single pathway can control both population maintenance and cell composition: stimulating proliferation is not sufficient if the resulting cell differentiation balance is wrong. Stromal signals are essential in vivo, and Paneth cells provide additional local support in small intestine; the colon maintains stem cells without a small-intestinal Paneth-cell arrangement. Niche dependence cannot therefore be equated with dependence on one invariant supporting cell type.
The adult organ is dynamically stable rather than cellularly static. A stem-cell clone can expand while neighbouring stem-cell clones disappear through neutral drift, with the total compartment maintained.[ref]
Intestinal crypt homeostasis results from neutral competition between symmetrically dividing Lgr5 stem cells by Hugo J. Snippert and others. Multicolour clonal tracing and neutral-drift analysis
At the organ level, sustained excess production generates expansion or neoplasia; excess loss causes barrier failure. Development deliberately changes total cell number, surface area and proportions over time, whereas adult maintenance constrains their long-term averages. Nevertheless, adult tissue homeostasis remains responsive to feeding, microbes, immune signals and injury, and is not a completely fixed endpoint.Experimental models expose both continuity and differences. A single sorted Lgr5 positive cell can produce a self-renewing intestinal organoid containing organized differentiated progeny in a suitable matrix and supplied growth factors. This establishes epithelial self-organization under defined conditions, not niche independence in the absence of extracellular signals: the medium replaces important niche functions.[ref]
Single Lgr5 stem cells build crypt-villus structures in vitro without a mesenchymal niche by Toshiro Sato and others. Single-cell cultures, lineage organization and defined culture requirements
Embryonic explants retain the mesenchyme needed to study villus patterning, while adult intestinal organoids are especially useful for stem-cell maintenance and lineage allocation. Neither alone reproduces an intact organ's circulation, innervation, immune environment and longitudinal regionalization.Finally, injury reveals an important bridge between development and maintenance. cell fate plasticity can restore missing stem cells, so the normal adult lineage flow is not an irreversible restriction of all descendants. Committed progenitor cells can recover stem-cell function under particular injury conditions, but this does not establish that all mature villus cells routinely do so. A decisive comparison uses stage-specific lineage tracing, matched marker analysis and timed pathway perturbation, measuring architecture and functional output as well as cell proliferation. Development and adult renewal reuse molecular machinery while differing in tissue geometry, developmental competence and the direction of net population change.
Past exam of the zoology course of the University of Cambridge 2025 Paper zl6 1 Solution by Codex 0 2026-10-20
Codex 0 2026-10-20The central task is to measure the cellular events that precede a branch, then perturb those events while preserving cell viability and organ identity. Similar final trees can arise through very different combinations of cell proliferation, cell migration, cell intercalation, cell shape change and lumen formation. I would therefore begin with an unbiased developmental description rather than assume that the organ uses the programme of a familiar vertebrate organ.
First establish a reproducible staging series from the unbranched primordium to the mature organ. Use serial sections and whole-mount confocal microscopy to distinguish epithelium, surrounding mesenchyme, extracellular matrix, nerves and blood vessels. Validate candidate epithelial cell and cell polarity markers by their localization and sequence rather than assuming that mammalian antibodies cross-react. A fluorescent luminal tracer, introduced without excessive pressure, would establish which spaces are continuous. Reconstruct the organ in three dimensions: an apparent bifurcation in a projection might instead be two crossing tubes or a fusion. Quantify organ volume, epithelial cell number, branch order, tip number, segment length and diameter, branch angle and timing. Distinguish lateral budding, tip bifurcation and branch fusion. The mouse lung illustrates the value of recording a branch genealogy: a complicated tree can be decomposed into reproducible local branching modes, but this is a methodological precedent, not evidence that the new species uses the same modes.[ref]
The branching programme of mouse lung development by Ross J. Metzger and others. Developmental reconstruction and identification of local branching modes
Next establish intact-animal live-cell imaging, preferably with light-sheet fluorescence microscopy if optical access allows it, and a complementary explant culture containing both epithelium and mesenchyme. Match temperature, salinity, oxygenation and developmental timing to the animal. Compare cultured and intact organs for branch rate, geometry, marker expression and cell death. Introduce membrane and nuclear fluorescent proteins at low expression and validate that imaging, immobilization and labels do not change development. Acquire full three-dimensional time series frequently enough to resolve division and neighbour exchange. Track nuclei and segment cell boundaries, manually auditing difficult divisions and branches. Express movement relative to the local tissue, so passive displacement by growth is not mistaken for active cell migration.
Measure separately the sources of tissue expansion. Short DNA synthesis labeling with EdU pulses locate DNA replication, pulse-chase experiments reveal subsequent displacement, and direct imaging records completed cytokinesis. A high mitotic fraction alone cannot establish rapid cell production because a prolonged mitosis also raises that fraction. Measure cell volume to distinguish cell growth from cell proliferation, and use a validated caspase reporter plus morphology to detect apoptosis or cell extrusion. For an explicitly bounded region, the bookkeeping identity is , where counts completed divisions in the region, deaths and live-cell entries and exits across its boundary. This checks whether tracked behaviours explain the measured cell-number change; lumen inflation or stretching can enlarge the organ without increasing .
Sparse permanent lineage tracing or local photolabelling before branch initiation would test whether tip and stalk populations are stable or exchange. Label a tip, a flank and a prospective cleft separately and follow their descendants. Do tip cells remain leaders, do flank cells feed the tip, or does an initially broad patch partition into daughter branches? Image oriented cell division, cell elongation, protrusions and junction turnover alongside branch emergence. A division aligned with a tube is only suggestive: track daughter positions and test whether changing the orientation changes elongation. Quantify neighbour exchanges to identify cell intercalation. In the fly trachea, microsurgery and genetic experiments showed that migrating tips generate tension that promotes stalk rearrangement, illustrating why seeing intercalation does not by itself show that it supplies the primary force.[ref]
Tip-cell migration controls stalk-cell intercalation during Drosophila tracheal tube elongation by Emmanuel Caussinus and others. Genetic and microsurgical tests of tip-generated tension
Then make acute, staged causal tests. Transiently inhibit the cell cycle after specification, verify suppression of completed divisions, and ask whether existing tips still extend or new branches initiate. Independently perturb actomyosin contractility, cell adhesion or a candidate migration regulator identified by the movies. Use short observation windows before generalized disorganization, and quantify cell number, apoptosis, cell polarity and organ markers in parallel. If division inhibition stops volume increase but preserves new clefts, proliferation supplies material without necessarily positioning clefts. If contractility inhibition abolishes clefts before cell number changes, a shape-generating role becomes plausible. Local laser ablation of a tip, a stalk junction or adjacent matrix, with sham irradiation controls, can test force transmission; recoil reports pre-existing load relative to resistance, not an absolute force without a mechanical model.
Use RNA interference for candidate screening and independent CRISPR genome editing alleles for confirmation. Require at least two independent targeting reagents, non-targeting and injection controls, quantitative target depletion, and rescue with a targeting-resistant functional allele. Inducible or mosaic perturbation, where technically achievable, separates an organ-specific requirement from an earlier embryonic defect. Mix labelled mutant and normal cells to distinguish a cell-autonomous defect from altered neighbouring signals or matrix. Separate epithelium and mesenchyme, recombine control and perturbed partners, and test matrix composition or localized candidate growth-factor delivery only after confirming that separated tissues remain viable. Use single-cell RNA sequencing and spatial expression to nominate pathways such as FGF signalling, but treat expression as a hypothesis generator rather than proof of behaviour.
Finally compare explicit alternative models of branching morphogenesis against held-out movies: localized cell production, directed collective movement, active rearrangement, or growth constrained by the surrounding matrix. Each should predict both branch geometry and the observed cell trajectories, and its response to a spatially restricted perturbation. Randomize treatment, blind segmentation and use animals from independent clutches as biological replicates; many cells within one animal do not replace independent animals. The strongest outcome is a causal chain from molecular perturbation to altered cell behaviour to altered branch geometry, supported by rescue and by measurements showing that general developmental delay cannot explain it.
Past exam of the zoology course of the University of Cambridge 2025 Paper zl3 6 Solution by Codex 0 2026-10-20
Codex 0 2026-10-20Conflicts are reduced by changing who benefits from cooperation, constraining opportunities for selfish success, or imposing costs on exploiters. The same logic operates between organisms and inside them, but the units that reproduce and transmit differ. Resolution need not mean eliminating all conflict or giving every participant its preferred outcome: it can be a stable compromise, suppression by a powerful party, or a continuing arms race.
An evolutionary conflict exists when different inherited strategies or replicating lineages favour different outcomes. Between organisms, individuals may disagree over resources, mating or contributions to a shared activity. Within an organism, cell lineages can gain from proliferating at their neighbours' expense, and genes can gain a transmission advantage that harms the rest of the genome. A common environment or membership of one body does not guarantee identical interests.
Between organisms, alignment can make restraint individually worthwhile. Genetic relatedness can reward benefits to relatives through inclusive fitness; repeated interaction can link current help to later returns; and partner choice can make productive cooperation a condition of continued association. Reliable exchange can also make a partner's survival directly valuable. None of these mechanisms requires conscious agreement. They work only where their gains outweigh the available selfish alternative, including the costs of assessment and enforcement.
Conditional allocation supplies another route. In soybean experiments, preventing rhizobial nitrogen fixation reduced bacterial reproductive success, while physiological measurements implicated reduced oxygen supply to non-fixing nodules. This supports host control that makes poor service costly to the symbiont. The treatment forced noncooperation in an otherwise cooperative strain: it tests the consequences of service failure, rather than demonstrating the evolutionary origin of a particular cheating mutation.[ref]
Host sanctions and the legume-rhizobium mutualism by E. Toby Kiers and others. 2003, nitrogen-free atmosphere treatment and nodule responses
Social insects show how relatedness and enforcement interact without making a colony conflict free. Workers can produce haploid sons, creating disagreement over male production. With a sufficiently multiply mated queen, a worker may be more related to queen-produced males than to the average other worker's sons. Experiments in honeybees found strong discrimination against worker-laid male eggs, supporting worker policing. The result establishes differential treatment of eggs; relatedness and colony productivity are possible selective benefits and must be evaluated rather than assumed equivalent.[ref]
Worker policing in the honeybee by Francis L. W. Ratnieks and P. Kirk Visscher. 1989, genetic incentives and experimental egg discrimination
Within multicellular organisms, common descent changes the baseline. Development from a single-cell bottleneck normally makes most cells close genetic relatives and links their lineage's long-term transmission to successful reproduction of the organism. Germline-soma differentiation further restricts the routes by which a proliferating somatic lineage can reach future generations. These features help explain extensive cellular cooperation, but they are incomplete protection: somatic mutation can create a clone that grows faster within the body even while lowering host survival or reproduction.
Cell-cycle regulation, DNA-damage responses, apoptosis, tissue architecture and immune responses can restrict such expansion. Some mechanisms remove damaged cells; others reduce opportunities for spread or prevent extra divisions from translating into transmission. Their developmental and maintenance functions mean that they should not all be described as adaptations exclusively for cancer suppression. Cancer demonstrates that the constraints can fail, especially when selection on the organism is weak at ages after most reproduction.
Apoptosis and cell competition are also not automatically measures of collective welfare. In experimental Drosophila tissues, higher Myc expression made clones eliminate lower-Myc neighbours and expand at their expense. This showed that a process involving elimination of neighbouring cells can be exploited by a locally successful lineage. It cautions against labelling whichever cells win a contest “best for the organism.”[ref]
dMyc Transforms Cells into Super-Competitors by Eduardo Moreno and Konrad Basler. 2004, mosaic tissues, neighbour elimination and clonal expansion
Genetic conflict can persist even when cells descend from one zygote, because loci may have different transmission rules. A sex-linked meiotic driver can increase its own representation by impairing gametes carrying the alternative chromosome. Autosomal alleles can instead favour restoration of a more balanced transmission system. In Drosophila simulans, genetic and molecular work identified the autosomal suppressor not much yang, which suppresses an X-linked sex-ratio distorter; cytological work connected distortion to failure of Y-bearing sperm maturation. This is a concrete case of a genomic countermeasure, rather than an assumption that Mendelian inheritance is intrinsically immune to selfish elements.[ref]
A sex-ratio Meiotic Drive System in Drosophila simulans. I: An Autosomal Suppressor by Yun Tao and others. 2007, suppressor characterization and sperm-development evidence
The comparison reveals two common principles. First, common transmission can align interests, as in relatives, vertically transmitted symbionts and clonally developing cells. Second, discrimination can make selfish strategies less profitable, as in partner sanctions, worker egg removal and suppression of a driver. Compartmentalization can help target the responsible partner or lineage, but its effect depends on scale: a compartment founded by one symbiont may reduce within-compartment mixing while still allowing competition among host compartments.
There are also important differences. Separate organisms can often leave, switch partners or use outside resources, so the costs of exit shape bargaining and partner choice. An ordinary somatic cell has few such reproductive alternatives and is usually integrated into a developmentally specified body. Genes inside that cell cannot choose partners in the behavioural sense, but recombination, linkage and differential transmission change the selection acting on suppressors. At either scale, suppression can select for evasion, producing continuing counteradaptation rather than permanent harmony.
A successful explanation therefore specifies the competing units, their routes of transmission, the benefit of the proposed control mechanism, and the level at which success is measured. More offspring, more surviving symbionts, a larger clone and greater representation of one chromosome are different outcomes. Conflicts are resolved to the extent that mechanisms make the lower-level selfish alternative less successful relative to its competitors; neither organismal organization nor social cooperation is evidence that the underlying conflict has vanished.
Past exam of the zoology course of the University of Cambridge 2025 Paper zl3 5 Solution by Codex 0 2026-10-20
Codex 0 2026-10-20Dependence evolves when a partner becomes a sufficiently reliable part of the environment that specialization on its services outcompetes maintaining an autonomous alternative. Reciprocal evolutionary change requires additional evidence. Ecological interdependence, obligate symbiosis and coevolution describe different properties: present-day benefit, inability to persist without assistance, and reciprocal heritable responses to selection, respectively.
An association can begin with incidental benefits. One species releases metabolic products, modifies habitat or consumes a toxin; another uses the altered environment. Initially neither partner need have evolved a service for the other. Repeated association can favour increased access to that benefit, spatial attachment or mechanisms that exchange complementary resources. Metabolic cross-feeding may arise from waste uptake before either producer becomes dependent on a particular recipient. This route requires no foresight and does not imply that the interaction started as costly altruism.
Once a service is sufficiently reliable, retaining an expensive redundant function may yield little advantage. Adaptive gene loss can then make the recipient dependent. Neutral deterioration under relaxed selection is another possible route, particularly when small populations and transmission bottlenecks weaken purifying selection. These explanations have different predictions about costs and selection and should not be conflated: a missing gene is not evidence, by itself, that losing it was adaptive. Moreover, dependence is conditional on the environment. A lineage unable to grow alone in one natural setting may grow without its usual partner when the missing resource or protection is experimentally supplied.
Experiments with Prochlorococcus illustrate this distinction. The cyanobacterium is vulnerable to extracellular hydrogen peroxide, and co-culture with peroxide-removing Alteromonas protected cells and enabled growth at low densities. Removing the surrounding microbial community also altered peroxide accumulation in seawater assays. These results establish an ecological dependence on a diffusible protective service in the tested conditions. They do not demonstrate that one specific helper species must be present, that helpers require Prochlorococcus in return, or that gene loss and reciprocal adaptation were observed evolving during the experiment.[ref]
Dependence of the Cyanobacterium Prochlorococcus on Hydrogen Peroxide Scavenging Microbes for Growth at the Ocean's Surface by J. Jeffrey Morris and others. 2011, peroxide measurements, co-culture and growth experiments
Reciprocal specialization can make dependence bilateral. If each partner increasingly relies on a different product or function supplied by the other, selection can favour complementary investment and reduced redundancy. Inherited association strengthens that feedback: successful host reproduction also transmits symbionts, so investment in host function can improve symbiont transmission. Vertical transmission and physical compartmentalization can therefore align some fitness consequences. They do not make interests identical, because symbionts can still compete within hosts and hosts can favour reduced costs of support.
Aphids and Buchnera aphidicola provide a strong example of a highly integrated association. The sequenced Buchnera aphidicola genome has extensive losses but retains pathways associated with essential amino-acid provision, consistent with nutritional complementation of the aphid's diet. The bacterium depends on the host-associated setting, while the host uses its biosynthetic contributions. This pattern supports derived specialization and loss of autonomy; the genome alone does not establish every metabolite exchanged or directly reconstruct the order of historical evolutionary changes.[ref]
Genome sequence of the endocellular bacterial symbiont of aphids Buchnera sp. APS by Shuji Shigenobu and others. 2000, reduced genome and retained biosynthetic functions
Dependence can also arise through repeated behavioural or ecological specialization rather than physical integration. A pollinator can specialize on a floral resource, or a predator on a particular prey. The affected partner may then evolve recognition, defence or counter-exploitation. Such interactions may remain facultative, asymmetric or antagonistic. Conversely, obligate association can arise through one lineage's losses while the other changes little. Thus the intensity of current dependence does not measure the amount of reciprocal evolution.
Coevolution requires each lineage to alter selection on the other, with a heritable response in both. A functional match between two traits is insufficient: both could have adapted to the same abiotic environment, one could have tracked the other, or different partners could produce the same match. An association might also result from ecological sorting of already compatible types. Immediate behavioural adjustment or altered gene expression is phenotypic plasticity unless an inherited change in the response itself is demonstrated.
Experimental host-parasite evolution gives a clearer test. In replicated populations of bacteria and bacteriophages, temporal comparisons of bacterial resistance and phage infectivity demonstrated reciprocal escalation, with divergence among replicate populations. Here changes in the antagonist's traits change the selective environment confronting the other lineage. This is evidence for an antagonistic arms race rather than merely a close ecological association. It also shows why coevolution is not restricted to beneficial partnerships.[ref]
Antagonistic coevolution between a bacterium and a bacteriophage by Angus Buckling and Paul B. Rainey. 2002, experimental resistance-infectivity dynamics and between-population differentiation
For a mutualism, reciprocal-transplant experiments can cross evolved hosts with ancestral and evolved symbionts, measuring both parties' performance in a common environment. Parallel evolution without the partner and controls for adaptation to the culture medium help isolate partner-mediated selection. In natural systems, time-shift assays, reciprocal genotype combinations and evidence that relevant traits affect partner fitness strengthen an inference; simple correlations and matching phylogenies remain vulnerable to shared environmental or transmission histories. Diffuse coevolution involving several interchangeable partners is possible and need not produce a one-to-one species pair.
The result may be complementary specialization and increasingly integrated reproduction, but stability is not guaranteed. Cheaters, changing environments, loss of partners and altered transmission can destabilize even an obligate association. The transition from incidental benefit to dependence is therefore explained by the relative costs of autonomy and association; the transition to coevolution is established only when reciprocal selection and heritable responses are demonstrated.
Past exam of the zoology course of the University of Cambridge 2025 Paper zl3 4 Solution by Codex 0 2026-10-20
Codex 0 2026-10-20Relatedness is not required when responding to others yields a sufficient direct benefit, and coordination need not begin as costly altruism. Coordinated behaviour means that individuals adjust the timing, position or type of their actions relative to others. Cooperation concerns benefits provided through an interaction, while evolutionary altruism specifically imposes a direct fitness cost on the actor. Confusing these categories makes unrelated coordination appear harder to explain than it is.
Consider animals travelling together. Matching a neighbour's direction can reduce an individual's predation risk or help it reach food. Both the responder and the neighbour may benefit immediately; no deferred repayment or kin recognition is necessary. Likewise, complementary hunters can each increase their own chance of capture by responding to another's actions. The relevant condition is that the expected direct return to the response exceeds its costs, relative to available alternatives. That condition depends on ecology, not merely on whether companions share genes.
A clear interspecific example is joint hunting by groupers and giant moray eels, which cannot be close genetic relatives. Field observations documented nonrandom associations, grouper recruitment signals and benefits to both partners. Their different hunting modes expose prey that could evade either hunter alone. Each captured prey item is swallowed by its captor, limiting disputes over division of a carcass. The study supports a direct-benefit mechanism; it does not require alternating favours or prove that every recruitment signal evolved specifically in that association.[ref]
Interspecific communicative and coordinated hunting between groupers and giant moray eels in the Red Sea by Redouan Bshary and others. 2006, associations, recruitment and complementary hunting modes
Simple response rules can make individually advantageous actions fit together. Attraction, alignment, avoidance and following informed individuals can generate collective movement without central control. A quorum response makes commitment more likely after enough others act, potentially preventing one mistaken individual from drawing the whole group into danger. Such proximate rules still need an evolutionary explanation: heritable differences in responsiveness must affect expected survival or reproduction in the environments where the rule is expressed.
Experiments with three-spined sticklebacks used moving replica fish to manipulate apparent social information. Larger groups under perceived risk were less readily led by a single replica than solitary fish, and nonlinear response models explained these decisions better than simple proportional copying. Simulations linked these rules to improved decisions under specified assumptions. The experiment establishes a plausible coordination mechanism; actual lifetime fitness gains and the historical selection of its parameters remain separate questions.[ref]
Quorum decision-making facilitates information transfer in fish shoals by Ashley J. W. Ward and others. 2008, replica-fish experiments and decision models
The strategic problem also depends on the payoff matrix. In a coordination game, joining a hunt can be a best response when others join, while acting alone is better when nobody else participates. Shared cues, recruitment signals and learned conventions can move a group toward the mutually beneficial equilibrium. Here the difficulty is reaching or maintaining compatible choices. In a prisoner's dilemma, by contrast, withholding a contribution pays better against either partner action in a one-shot encounter. An account of coordinated hunting must establish which incentives actually apply rather than assume every group activity is a public-goods dilemma.
When cooperation does carry an immediate cost, direct reciprocity can make future consequences matter. In a deliberately simple repeated donation game, giving costs and benefits a partner by . If encounters continue with probability , perpetual mutual cooperation yields . Defecting once against a cooperator yields if it then triggers permanent noncooperation. Cooperation is preferable against that deviation whenThis is a conditional comparison under recognition, reliable observation and the specified retaliation rule. It is not a universal threshold for animal cooperation, nor does it show that a rare cooperative strategy can always invade an uncooperative population. Primary repeated-game modelling and computer tournaments established how such contingent interactions can sustain cooperation under suitable conditions.[ref]
The evolution of cooperation by Robert Axelrod and William D. Hamilton. 1981, theoretical model and strategy tournament
Other mechanisms need not involve repayment by the same individual. Partner choice can reward useful collaborators through access to future interactions; leaving an unproductive association can impose an opportunity cost on a defector. Reputation can alter future access to different partners. Partner fidelity feedback occurs when helping a partner increases the actor's future benefits because that partner survives or becomes more productive. These mechanisms require appropriate encounter structure, information and opportunities to choose; naming them is not evidence that a particular species uses them.
Evolutionary policing or partner sanctions can change the returns to exploitation. As a mechanistic example involving unrelated partners, soybean experiments prevented a normally fixing rhizobial strain from fixing nitrogen by changing its atmospheric supply. Reduced bacterial reproductive success and oxygen-supply measurements supported a host-sanction interpretation. This shows how conditional resource allocation can favour service provision without kinship, although it is not by itself an example of synchronized animal movement or proof of the historical origin of the interaction.[ref]
Host sanctions and the legume-rhizobium mutualism by E. Toby Kiers and others. 2003, experimental prevention of nitrogen fixation and symbiont performance
Coordination can consequently evolve through several routes: immediate mutual benefit, stable contingent exchange, partner assortment, or changed incentives imposed by others. Learning can implement or transmit successful rules, while genetic evolution shapes learning capacities and costs. These explanations are compatible with multilevel descriptions of selection, but a claim that groups benefit is insufficient unless the process maintaining the relevant individual strategies is specified. Effective groups of unrelated individuals emerge when responding and contributing are viable strategies in their actual ecological and social setting.
Past exam of the zoology course of the University of Cambridge 2025 Paper zl3 3 Solution by Codex 0 2026-10-20
Codex 0 2026-10-20Consistent individual differences can bias who leads, works, reproduces or takes risks, but a social role is usually produced jointly by an individual's traits and its social environment. A stable pattern of participation is not necessarily a fixed genetic caste, and observed specialization is not automatically evidence of superior skill.
First distinguish the measurements. Animal personality denotes repeatable among-individual differences in behaviour; a behavioural syndrome is a correlation across behavioural contexts. A social role describes an individual's contribution or position in a particular group, such as initiating travel or carrying brood. A member can repeatedly occupy a role because of morphology, age, nutritional state, information, experience or treatment by others. Some of these causes change predictably during life, so consistency over a short observation window need not imply lifelong specialization.
One proximate route is variation in behavioural response thresholds. A worker with a lower threshold for responding to brood demand begins care sooner; a hungry fish leaves shelter sooner; an informed animal initiates movement toward food. Once a member acts, it can reduce the stimulus facing others. That negative feedback helps partition labour even when initial differences are small. Conversely, practice or social reinforcement can lower the actor's future threshold or increase others' reliance on it, amplifying small initial differences into persistent roles. These are testable mechanisms, not reasons to assume that a group allocates tasks deliberately.
Animal leadership illustrates the importance of relational effects. In experimental pairs of three-spined sticklebacks, researchers first measured willingness to leave cover, then paired fish and modelled their movements. Relatively bold fish more often initiated joint trips, but both partners adjusted to the other's movements. Leadership therefore arose from differences in responsiveness as well as spontaneous initiation. It was neither simply the most active fish's solitary phenotype nor evidence that followers had surrendered all influence.[ref]
Social feedback and the emergence of leaders and followers by Jennifer L. Harcourt and others. 2009, individual assays, paired trials and movement-state model
A second route is division of labour based on developmental or physiological differences. Body size can alter the mechanical returns to defence or transport; age can alter experience, residual lifespan and the cost of risky work. Members can thereby specialize on tasks for which their relative performance is better, even if another individual performs more tasks better in absolute terms. However, morphology may also constrain a role rather than represent an adaptation specifically for the present task, and an age pattern alone does not identify its endocrine or social cause.
Honeybee experiments provide evidence for that distinction. Rearing workers in groups of different sizes and transplanting older bees into otherwise forager-deficient colonies altered endocrine and behavioural development. Young workers could begin foraging unusually early under changed colony conditions. These manipulations show that worker-worker interactions affect age polyethism; age is not an independent clock that irreversibly assigns each bee its task.[ref]
Honeybee colony integration: worker-worker interactions mediate hormonally regulated plasticity in division of labor by Z. Y. Huang and Gene E. Robinson. 1992, group-rearing and older-worker transplant experiments
Roles can be maintained through feedback without being individually optimal in every context. Repeated experience can improve information about a particular location, while repeated exclusion from reproduction can make helping the best available option. A dominance hierarchy can distribute access to food or breeding, but rank may reflect competitive constraints rather than efficient allocation. A subordinate's increased work may therefore result from limited alternatives or coercion, not from a freely chosen cooperative specialization. These possibilities predict different changes after removing dominant members or opening breeding opportunities.
At the group level, complementary tendencies can reduce duplicated effort, switching costs and interference. A mixture of initiators and responsive followers can exploit information that a uniformly cautious group would not use; different thresholds can spread effort across tasks. Yet too many risk-taking initiators may fragment a group, while excessive following may create dependence on poorly informed leaders. The effects therefore depend on composition, task demand and environmental variation. A positive association between behavioural diversity and performance is not enough to establish that selection maintains that diversity: group size, resource supply and group age may influence both.
Nor does specializing necessarily make a worker an expert. In Temnothorax albipennis, measurements across several tasks found that individual specialization did not predict higher task efficiency, and much work was not performed by the most efficient workers. This rejects a simple specialization-equals-skill explanation in that study. It leaves other possible benefits, including task coverage and reduced switching or coordination costs, to be tested independently.[ref]
Specialization Does Not Predict Individual Efficiency in an Ant by Anna Dornhaus. 2008, individual task performance and allocation of labour
Persistent differences can themselves be socially maintained. An individual repeatedly treated as a leader obtains more opportunities to lead; a member repeatedly excluded from one task acquires less experience in it. Social niche specialization can thus stabilize a distribution of roles through feedback between behaviour and partner responses. At the same time, phenotypic plasticity permits replacement after a worker or leader disappears. A group can display stable role proportions while its individual members change roles, so stability of organization should not be confused with rigidity of membership.
A causal study should follow identified individuals across repeated contexts, estimate behavioural repeatability after accounting for age and state, and measure partners' responses. Cross-fostering, standardized hunger manipulations, group-composition changes and member removals can distinguish pre-existing propensities from social induction. Performance should be measured separately from time allocated to a task, and group productivity separately from each member's reproductive success. These distinctions also expose cases in which a role benefits others while imposing costs on its occupant.
Consistent differences therefore supply biases from which social organization can emerge, but the resulting roles are conditional, relational and often reversible. The strongest explanation links an individual trait to a response rule, shows how interactions turn that rule into a role, and tests the consequences for both the individual and the group.
There are unlisted articles, also show them or only show them.