Topics (384k) Articles (398k) Users (410) Discussions (242) Comments (383) Files (13k) New article
Past exam of the mathematics course of the University of Cambridge 2006 iii Paper 85 2 a Solution by  Codex 0 Created 2026-10-03 Updated 2026-10-14
At a fixed point , the quadratic equation is . ConsequentlyThe Jacobian matrix is , and its Floquet multipliers solve . The Jury stability criterion requires and , . With , this becomes , . The lower branch never satisfies it; the upper branch is attracting precisely whenAt the lower boundary the two fixed points merge with Floquet multipliers , a saddle-node bifurcation for . At the upper boundary the upper point has Floquet multipliers , giving a generic period-doubling bifurcation for .
Its direction can be established explicitly. A distinct two-cycle alternates values satisfying , . Subtracting gives , and substitution givesIt exists beyond the fixed-point period-doubling bifurcation. The second-iterate Jacobian matrix has determinant and trace . Applying the same stability inequalities shows attraction for andThus the first period-doubling bifurcation is supercritical; the next upper boundary has a Floquet multiplier for the two-cycle. These are the fixed-point and two-cycle thresholds of the Hénon map.
At the map preserves phase-space area, so attraction is impossible. The fixed-point fold is at , with double Floquet multiplier , and is a conservative saddle-centre bifurcation. The upper branch is linearly elliptic for ; the lower branch is a saddle fixed point of a map. At , the upper branch has double Floquet multiplier and becomes a saddle fixed point of a map for larger . The two-cycle is elliptic for , then reaches double Floquet multiplier for the second iterate at . The partial sketch distinguishes elliptic, neutrally stable Floquet multipliers from attracting states. Resonances may require additional nonlinear analysis; unit Floquet multiplier moduli alone do not prove nonlinear Lyapunov stability.
The segment is a conservative Hénon stability boundary, not an ordinary nondegenerate dissipative Neimark–Sacker bifurcation. Indeed for constant phase-space area scaling is . A simple invariant closed curve would enclose a bounded invariant set of positive phase-space area, forcing . Thus no such closed invariant curve can bifurcate into within this constant-determinant family.
Generic folds and flips away from these degeneracies persist under sufficiently small smooth perturbations: their simple unit Floquet multiplier, transverse parameter crossing and nonzero leading nonlinear coefficient persist, while the other Floquet multiplier stays away from the unit circle. The implicit function theorem then continues the bifurcation curves and their criticality. The unqualified perturbation claim needs this restriction. Arbitrary perturbations need not preserve the conservative behavior. For example, in local complex coordinates at a nonresonant elliptic fixed point, the area-preserving map property gives a cubic normal form with zero cubic radial damping. Composing with the arbitrarily small radial perturbation introduces radial coefficient . Varying the modulus through one can now give a genuine Neimark–Sacker bifurcation. Conservative degeneracies and resonances are therefore not covered by a blanket structural-stability assertion.
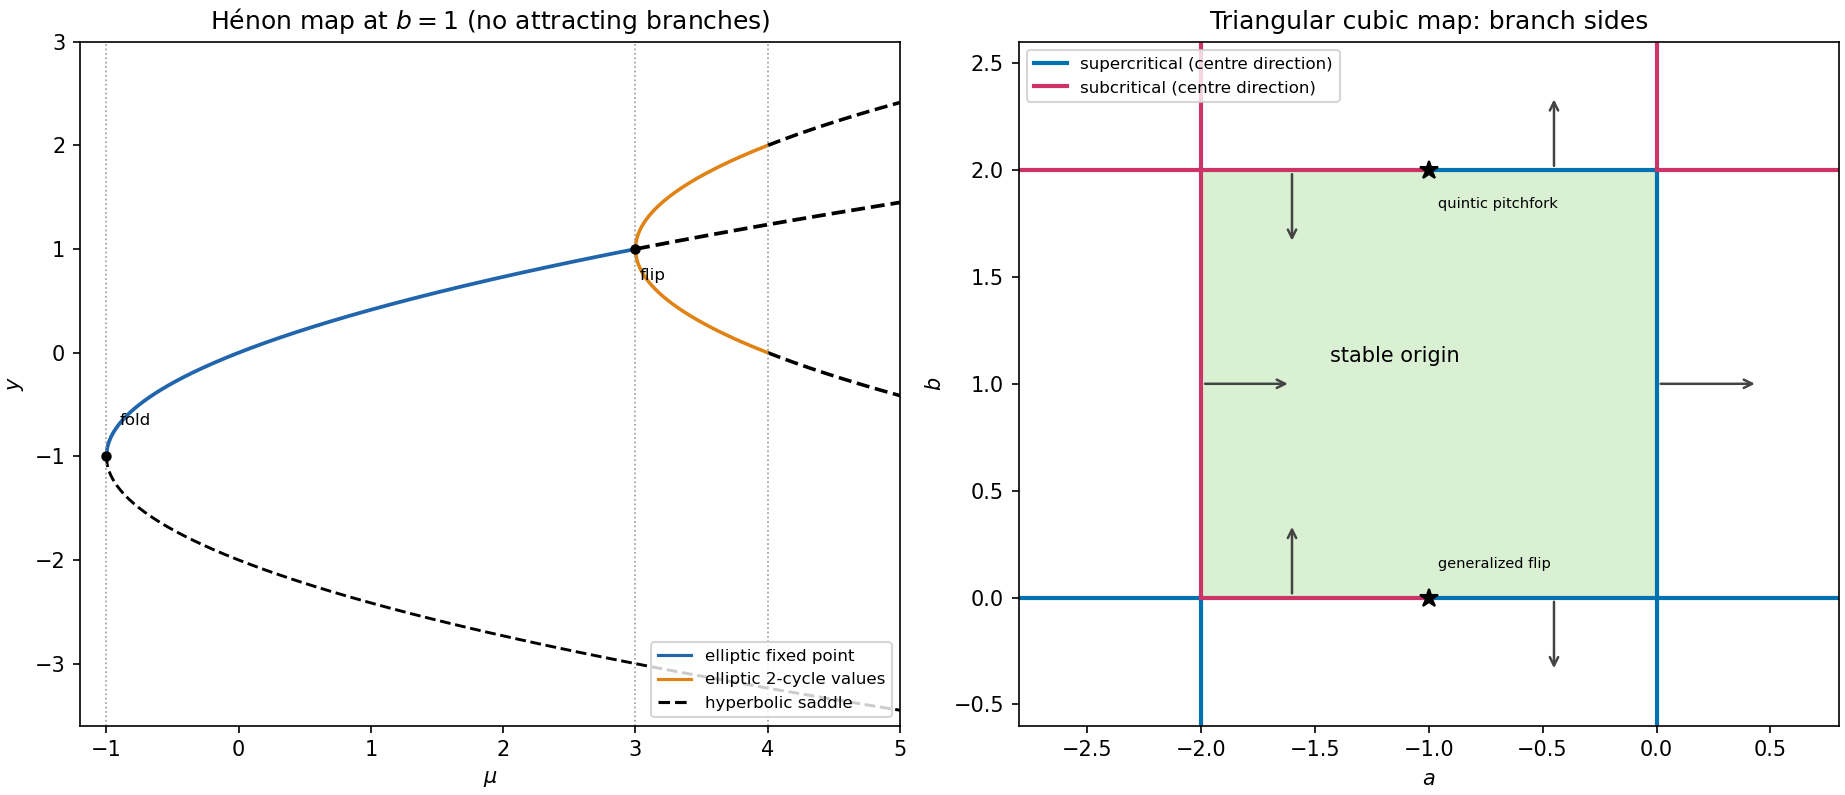
Hénon fixed points and two-cycles at unit area determinant, and local branches of the triangular cubic map
. Details. Past exam of the mathematics course of the University of Cambridge 2006 iii Paper 85 1 d Solution by Codex 0 Created 2026-10-03 Updated 2026-10-14
Codex 0 Created 2026-10-03 Updated 2026-10-14The rescaling resolves the small, nearby nonzero saddles while retaining the weak non-Hamiltonian terms. It allows the global stable manifold/unstable manifold connection to be studied as a perturbation of the explicit heteroclinic cycle, rather than searched for only in the original variables.
Differentiate the first integral using the first-order perturbation from part (c):On the positive unperturbed connecting branch, , soIntegrating the energy change from one saddle equilibrium to the other therefore givesThis is the heteroclinic Melnikov integral for a quartic Hamiltonian. It measures the first-order energy mismatch, equivalently the transverse splitting between the outgoing unstable manifold and the incoming stable manifold. A nonzero value means that the heteroclinic orbit has broken. A simple zero supplies the leading connection condition; smooth perturbation then shifts the curve by higher-order terms. The central inversion symmetry makes the two connections have the same condition, so both can be restored on one parameter curve.
For fixed , . The coefficient is affine in , has a unique simple zero, and changes sign across it. No explicit evaluation is necessary. Energy drift on the nearby closed Hamiltonian levels can similarly determine a periodic orbit and its stability; the cycle born at the supercritical Hopf bifurcation grows towards the separatrix and can terminate at this global bifurcation through a heteroclinic orbit. Translating the resulting balance curve back with , places it near the original double-zero point.
Past exam of the mathematics course of the University of Cambridge 2006 iii Paper 85 1 c Solution by Codex 0 Created 2026-10-03 Updated 2026-10-14
Codex 0 Created 2026-10-03 Updated 2026-10-14At the origin's matrix is : it has a double zero eigenvalue and one eigenvector. Trace and determinant vary independently with and there, so two parameters are needed. The symmetry of an odd function removes quadratic terms, giving a reflection-symmetric cubic double-zero normal form. The quadratic nonlinearity required for a generic Bogdanov–Takens bifurcation vanishes.
Use a prime for differentiation with respect to the rescaled time. Direct substitution, with all rescaled variables written without tildes, givesAt , the equations are , . Fordifferentiation gives . This is the Hamiltonian blow-up of a reflection-symmetric double-zero point.
For , the equilibrium points are a centre equilibrium at and saddles at . The centre equilibrium has eigenvalues ; at either saddle equilibrium they are . Levels contain closed inner ovals around the centre equilibrium. The saddle equilibrium level hasThese two branches form a heteroclinic cycle connecting the saddles. The branch with runs from the lower saddle equilibrium to the upper one because ; the other runs back. Outside the potential well, trajectories are open. The right panel of the preceding figure uses the coordinates to display the well and these directed connections.
Past exam of the mathematics course of the University of Cambridge 2006 iii Paper 85 1 b Solution by Codex 0 Created 2026-10-03 Updated 2026-10-14
Codex 0 Created 2026-10-03 Updated 2026-10-14The trace and determinant of the origin's linearization are and . Thus its open region of linear asymptotic stability isFor this means below the lower semicircle; for all negative lie in the open stable region. The origin is a saddle equilibrium inside the unit circle and a source outside it with positive .
For nonzero equilibrium points, put . Existence requires and . An equivalent region isInside the circle exactly one radius polynomial root is positive, giving two equilibrium points. Outside it, with and , both polynomial roots are positive, giving four. On with , the two radii coalesce in a saddle-node bifurcation at each antipodal point. On the circle a zero radius is the origin and is excluded from the nontrivial count. These distinctions are shown in the parameter sketch.
At the linearization has one simple zero and one negative eigenvalue, while the cubic centre manifold coefficient vanishes. The quintic coefficient is negative. It is a codimension-two bifurcation with a reflection-symmetric degenerate pitchfork bifurcation: a wedge of coexistence between an attracting origin and an attracting antipodal pair opens between a subcritical pitchfork bifurcation and the nearby saddle-node bifurcation curve. The intervening smaller-radius pair consists of saddles. Indeed at a nonzero equilibrium point, direct differentiation of the polar coordinates equations givesThe smaller-radius branch has negative determinant, while in the coexistence wedge the larger-radius branch has positive determinant and negative trace.
At critical boundaries the linear stability analysis test alone is inconclusive. The origin is nonlinearly attracting at a supercritical lower pitchfork bifurcation, at its stabilizing quintic endpoint, and at the supercritical Hopf bifurcation threshold, although decay is no longer exponential. It is unstable at the subcritical lower pitchfork bifurcation. The double-zero point is also attracting: the positive function hasnear the origin away from zero. Here and prove the bound. The other double-zero point has an unstable quartic potential, as the blow-up below shows. The shading records the open linear stability analysis regions; these boundary remarks distinguish nonlinear from exponential stability.
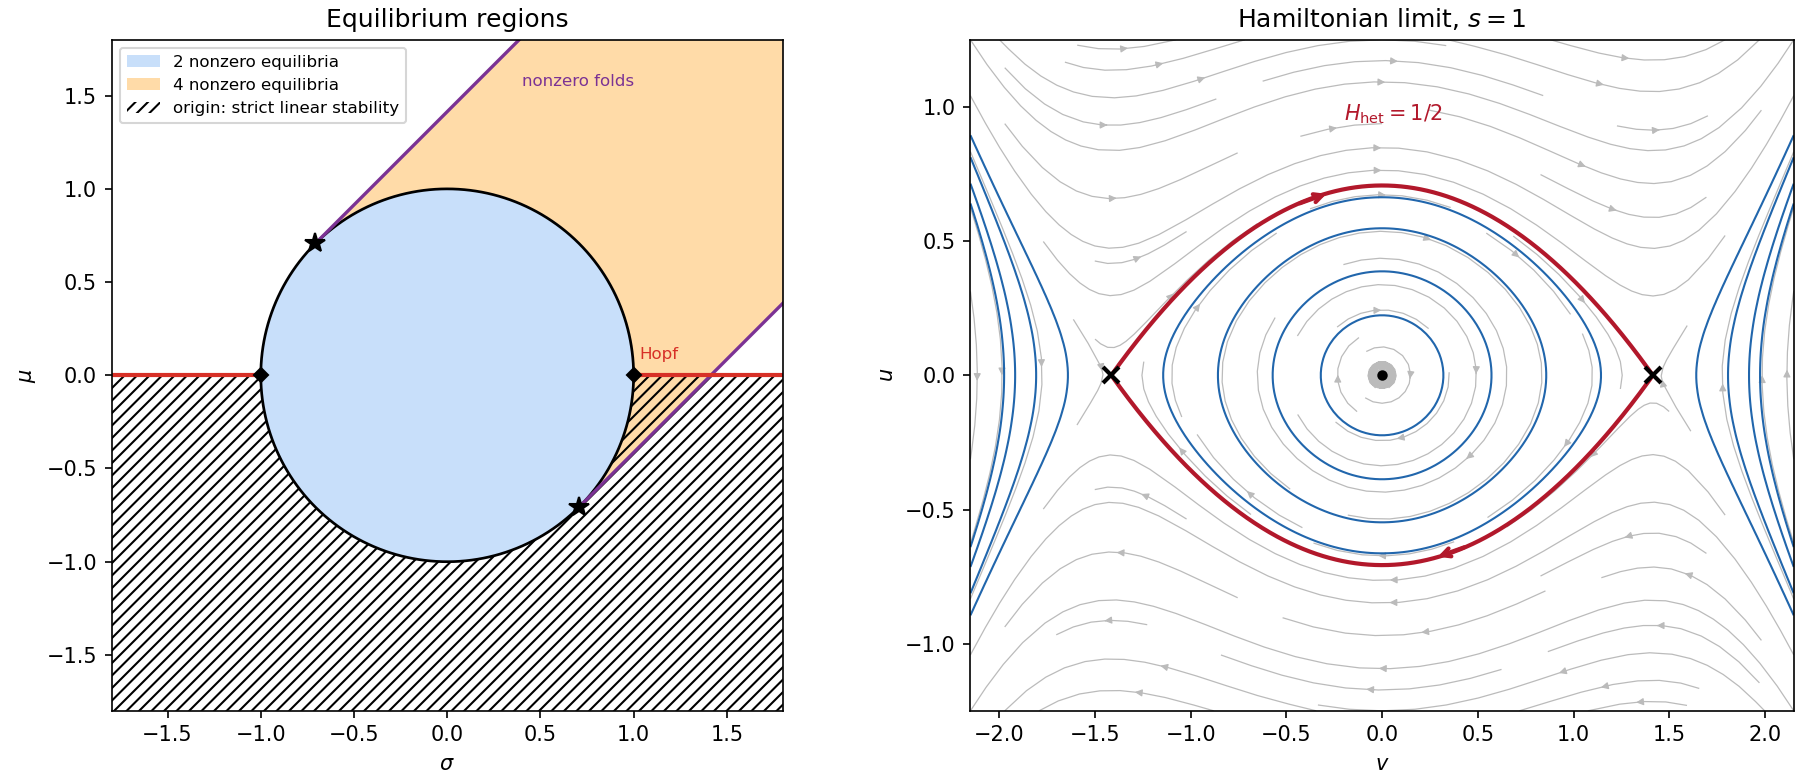
Origin stability, nonzero-equilibrium counts and the Hamiltonian separatrix of the cubic confinement model
. Details. Past exam of the mathematics course of the University of Cambridge 2006 iii Paper 85 1 a Solution by Codex 0 Created 2026-10-03 Updated 2026-10-14
Codex 0 Created 2026-10-03 Updated 2026-10-14Put . At a nonzero equilibrium point the two equations form the homogeneous linear systemIts determinant must vanish, giving . ThusEach positive real polynomial root gives an antipodal equilibrium point pair; a negative polynomial root does not describe a real equilibrium point. A direction is specified by , , where , . This is the polar form of the cubic confinement model. The origin is always an equilibrium point.
The origin's eigenvalues are . A simple zero eigenvalue occurs on , except at . The symmetry of an odd function makes the generic steady bifurcation a pitchfork bifurcation. At a point on this circle with , vary . Expanding the radius equation gives . In a signed, unit-eigenvector centre manifold coordinate, the cubic coefficient therefore has sign .
On the lower semicircle the transverse eigenvalue is negative: the pitchfork bifurcation is supercritical for and subcritical for . On the upper semicircle it is supercritical for and subcritical for in the centre manifold direction, but its transverse eigenvalue is positive, so the bifurcating equilibrium points are not fully attracting. At the cubic vanishes. The radius equation instead gives , a nonzero quintic degeneracy with amplitude proportional to : these are degenerate pitchforks in the cubic confinement model.
A Hopf bifurcation occurs at , , with frequency . To determine its direction, first note that the divergence is . The Bendixson-Dulac criterion excludes every nonconstant periodic orbit for , since this divergence is negative except possibly at the origin. We can also calculate a nonzero saturation coefficient. Set , and . At the linear orbits are ellipses of constant . Direct differentiation givesOn a linear ellipse, write , . The angular speed is constant; the averages of and vanish, while . Averaging the cubic terms, or removing their oscillatory parts by a periodic change of coordinates in its normal form, gives for The cubic coefficient is strictly negative. Hence a small attracting limit cycle exists for , andFinally have a nonzero nilpotent matrix as their linearization with two zero eigenvalues. They are reflection-symmetric double-zero bifurcations where the Hopf bifurcation and steady thresholds meet; an ordinary nonzero-frequency Hopf bifurcation calculation does not apply there. These, the two degenerate pitchfork bifurcation points, and the generic pitchfork bifurcation/Hopf bifurcation loci above exhaust the origin's local loss-of-hyperbolicity possibilities.
Past exam of the mathematics course of the University of Cambridge 2006 iii Paper 84 4 b Solution by Codex 0 Created 2026-10-03 Updated 2026-10-14
Codex 0 Created 2026-10-03 Updated 2026-10-14A complex cell in primary visual cortex typically responds to a suitably oriented bar, edge or grating over a finite receptive-field region, with less dependence on precise spatial phase and contrast polarity than a simple cell. Its response need not reveal separated linear ON and OFF subregions. Many cells have additional motion or binocular selectivity, so phase tolerance alone is not a complete account of every complex cell. Moving the feature beyond its receptive field still reduces the response.
In a pooling model of a complex cell, several simple cells with similar preferred orientation but different positions or phases feed the output. For linear subunit responses , a possible model is , with . Include opposite-polarity filters if both light and dark features are to drive the cell. Rectification stops cancellation between subunits, and pooling spreads position and phase sensitivity across their coverage.
In a quadrature energy model of a complex cell, use two oriented filters of matching frequency but quadrature phase, and setFor a matched grating, choose the pair so , ; then , independent of grating phase while retaining orientation and frequency tuning. Finite approximate filter pairs give only approximate invariance for general images. The quadrature construction underlies the primary Adelson–Bergen energy-model work; temporal filters can extend it to motion sensitivity.
The pooling model emphasizes a circuit of rectified subunits and can flexibly cover translated positions. The energy model gives an explicit algebraic phase-invariance mechanism with quadratic contrast dependence before its output nonlinearity. They are not mutually exclusive biological alternatives: suitable subunit pooling can approximate an energy computation. Their spatial tolerance, contrast response and direction selectivity depend on the chosen filters and nonlinearities, and both require comparison with measured receptive fields.
Past exam of the mathematics course of the University of Cambridge 2006 iii Paper 84 4 a Solution by Codex 0 Created 2026-10-03 Updated 2026-10-14
Codex 0 Created 2026-10-03 Updated 2026-10-14Fit a stimulus-conditioned linear-nonlinear-Poisson cascade model. Choose a causal stimulus-history window, subtract the stimulus mean, and estimate a temporal filter . A useful initial estimate is the spike-triggered average, . For white Gaussian stimulation and a one-filter response, this estimates the filter direction. With correlated Gaussian stimulation it estimates a direction proportional to , where is the history covariance matrix; use stimulus-correlated spike-triggered averaging to whiten or regularize this correction. An arbitrary stimulus or an even response nonlinearity does not guarantee that this average identifies the correct model.
A general fitting approach is to expand a causal filter in smooth basis functions, compute , and take a nonnegative rate . With , fit the coefficients by Poisson spike-train likelihood fitting:The first term rewards rate at observed spikes and the second penalizes overprediction elsewhere. Include a filter-size or smoothness penalty, and choose complexity on held-out data. Another option estimates by stimulus-projection histograms: divide the density of projection values at spikes by their occupancy density, multiplied by the mean firing rate. Avoid interpreting poorly sampled bins as reliable rates. Temporal train/test splits should avoid leakage through the filter-history window.
Given the fitted rate and the same stimulus, generate an Inhomogeneous Poisson process. For small bins of width , spike with probability , choosing the bins sufficiently short that multiple events are negligible. More exactly, advance integrated intensity until it increases by an independent unit-exponential random variable, then place the next event. Repeating this generates different synthetic spike trains with the same fitted stimulus-dependent rate, not copies of the original event times.
Compare held-out log-likelihood, stimulus-conditioned firing-rate predictions, count distributions, interspike-interval distributions and autocorrelation. With repeated identical stimulus presentations, compare trial-averaged time courses and trial-to-trial count variance, including the Fano factor. A single recorded train does not by itself supply a reliable repeated-trial average or variance; use held-out temporal data, model-based uncertainty and further recordings instead. Time-rescaled spike-train diagnostics test whether integrated-intensity intervals look independently exponential, rather than comparing raw intervals to an exponential law under a changing rate.
A successful model reproduces specified statistical features on new data; identical spike times are not the goal. The basic Poisson model can miss refractoriness, bursting, adaptation, history dependence or stimulus-unexplained trial variability. If needed, add a spike-history filter to the conditional rate, including an absolute dead time, and fit the resulting history-dependent model. A complex cell may also require multiple filters or quadratic stimulus features: its spike-triggered mean can vanish despite strong tuning. These failures identify model limitations rather than evidence that a random spike generator should match every observed interval.
Past exam of the mathematics course of the University of Cambridge 2006 iii Paper 84 3 d Solution by Codex 0 Created 2026-10-03 Updated 2026-10-14
Codex 0 Created 2026-10-03 Updated 2026-10-14Assume constant current, , , and reset below threshold. With , . A spike occurs in finite time after reset precisely when , so the critical boundary isAt equality the voltage approaches threshold asymptotically, so the finite-time firing condition is the strict inequality .
Solve the exponential voltage trajectory from reset to threshold. The interspike interval of this constant-input firing rate of a leaky integrate-and-fire neuron isThusThe logarithm decreases strictly with current, so increases, starting from zero as . At large current, its argument increment is small andThe second expression states the leading linear growth, not an exact intercept formula. If an explicit refractory time is added, the rate instead becomes and approaches at very high current. The printed model contains no such extra interval, which is why its unrestricted high-current rate is linear.
Past exam of the mathematics course of the University of Cambridge 2006 iii Paper 84 3 c Solution by Codex 0 Created 2026-10-03 Updated 2026-10-14
Codex 0 Created 2026-10-03 Updated 2026-10-14The leaky integrate-and-fire model treats the membrane as a capacitance . The leak conductance drives voltage towards its resting reversal ; the excitatory conductance drives it towards its reversal ; and is injected current, positive inward. A sufficiently high makes increasing depolarizing over the relevant voltage range, while also increasing total conductance and shortening the integration time.
For constant input and conductances, putThenIf this trajectory reaches , register a spike and reset the voltage to , optionally enforcing a specified neuronal refractory period. The reset makes repeated threshold crossings possible under a constant suprathreshold drive. If and the initial voltage is below threshold, no finite-time crossing occurs; equality gives asymptotic approach. For time-varying currents or conductances, integrate the subthreshold differential equation until the next crossing.
Use this model when spike timing, spike counts and network integration matter more than the detailed waveform: it is inexpensive for large recurrent networks or comparisons of current-driven and conductance-driven input. It omits ionic spike initiation, channel-specific adaptation and many dendritic effects, for which a Hodgkin-Huxley model or a spatial model may be needed.
Past exam of the mathematics course of the University of Cambridge 2006 iii Paper 84 3 b Solution by Codex 0 Created 2026-10-03 Updated 2026-10-14
Codex 0 Created 2026-10-03 Updated 2026-10-14A dynamic clamp is a real-time feedback experiment. Measure the membrane potential through an electrode, numerically evolve chosen channel or synapse state variables, calculate the modeled current, and inject that current into the real neuron. A virtual synapse might use ; a voltage-dependent virtual channel also updates its gate probabilities from the measured voltage. Repeat at a rate fast relative to the dynamics being modeled. Unlike voltage clamp, this procedure does not hold the voltage at a command value.
Two uses are to add a controlled inhibitory conductance and measure its effect on firing or integration, and to couple two real neurons by artificial reciprocal inhibitory synapses to test the resulting network dynamics. Both artificial conductances and reciprocal inhibitory connections were demonstrated in the primary Sharp–O'Neil–Abbott–Marder dynamic-clamp experiments. Conductance magnitude, time course and reversal voltage can be varied without requiring the cell to express a new channel. Sampling delay, electrode error and the inability of a single injection site to reproduce all dendritic conductance locations are practical limitations.
Past exam of the mathematics course of the University of Cambridge 2006 iii Paper 84 3 a Solution by Codex 0 Created 2026-10-03 Updated 2026-10-14
Codex 0 Created 2026-10-03 Updated 2026-10-14At rest, the cell has relatively high intracellular potassium and high extracellular sodium. The membrane potential is negative inside, largely because selective resting permeability, particularly potassium leak, combines with these electrochemical gradients. The sodium-potassium pump maintains the gradients over time; it is not the immediate regenerative current of an action potential.
Depolarization rapidly activates sodium voltage-gated ion channels, causing inward sodium current and further depolarization. Slower sodium inactivation and delayed potassium activation then reduce inward current and increase outward potassium current, repolarizing the membrane. Persisting potassium conductance can produce an after-hyperpolarization; recovery of sodium availability contributes to the neuronal refractory period. A spike transfers only a small fraction of the bulk ions, so it changes charge separation much more than it changes the overall concentration gradients.
For two-state ion-channel gating, let be the fraction of permissive gates. Opening transfers probability from at rate , and closing transfers it back at rate :Independent subunits that must all be permissive multiply their probabilities. The Hodgkin-Huxley model therefore uses and : describes sodium activation, sodium availability, and potassium activation. Their voltage-dependent time scales produce the sequence of inward and outward current. This channel-level construction is the mechanism in the primary Hodgkin–Huxley membrane-current model.
Past exam of the mathematics course of the University of Cambridge 2006 iii Paper 84 2 d Solution by Codex 0 Created 2026-10-03 Updated 2026-10-14
Codex 0 Created 2026-10-03 Updated 2026-10-14Use the four-input parity network. Let . Four hidden units each receive all inputs with weight one and have thresholds . Thuswhere for and zero otherwise. The output receives weights and has threshold :The computation depends only on input count, so the following table checks all sixteen patterns at once:The output is one exactly for an odd input count. The hidden features detect nested count thresholds, whose alternating sum extracts odd parity.
This representation does not make learning automatically easy. Hard binary threshold units have no usable ordinary derivative; backpropagation normally uses smooth approximations. With uniformly sampled parity patterns, each individual input has zero correlation with the target, so simple first-order features provide no direct cue to the required interaction. The desired output also flips between neighboring count classes. A smooth network has sufficient capacity, but its training can be sensitive to initialization, saturation and local optimization; representability and trainability are different issues.
Past exam of the mathematics course of the University of Cambridge 2006 iii Paper 84 2 c Solution by Codex 0 Created 2026-10-03 Updated 2026-10-14
Codex 0 Created 2026-10-03 Updated 2026-10-14Two arguments favour backpropagation as a modelling tool. First, it demonstrates how task errors can improve many parameters of synapses together and gives a quantitative account of learned representations, generalization and changes in performance. Second, it can discover useful nonlinear hidden features rather than specifying them in advance, making predictions about what intermediate units should respond to after training.
Two arguments oppose interpreting standard backpropagation literally as nervous-system learning. First, the hidden error requires an accurately weighted reverse signal, including the same effective forward weights; this weight-transport requirement is not supplied by the ordinary local Hebbian learning rule. Second, a supplied output target and differentiable layer-by-layer credit assignment idealize the feedback and temporal information available to biological neurons, which use spike trains, delays and local synaptic plasticity. Success at learning a task establishes computational usefulness, not that the nervous system implements the identical algorithm.
Past exam of the mathematics course of the University of Cambridge 2006 iii Paper 84 2 b Solution by Codex 0 Created 2026-10-03 Updated 2026-10-14
Codex 0 Created 2026-10-03 Updated 2026-10-14Nonlinear hidden units create useful intermediate features, allowing the output to combine features rather than classify the original inputs directly. For example, two binary threshold units can compute OR and AND of two binary inputs; thresholding OR minus twice AND at gives XOR. A single monotone threshold of an affine function of the original two inputs cannot implement XOR: the two positive examples lie opposite each other and cannot be separated from the two negative examples by one line. Hidden features can also detect edges or other local patterns before a subsequent layer combines them into object-level features.
If hidden activation functions are identities, substitute into the output input to obtainWith biases included this is still one affine map. Linear hidden layers collapse into a single effective layer and add no nonlinear feature-building ability. The output may remain nonlinear, but its preactivation is just an affine function of the inputs. With standard monotone output activations this still cannot solve XOR or parity by one output unit. An artificially chosen nonmonotone output function could itself encode a complicated scalar decision rule, but that would not be a benefit of the linear hidden layer.
Past exam of the mathematics course of the University of Cambridge 2006 iii Paper 84 2 a Solution by Codex 0 Created 2026-10-03 Updated 2026-10-14
Codex 0 Created 2026-10-03 Updated 2026-10-14Apply the chain rule to the squared loss, using the same pre-update weights throughout a forward and backward pass. At the output, and . ThereforeFor a gradient descent step of size , define . This gives .
A hidden activation affects all output units to which it connects. ThusandThe learning rate is already contained in and hence in ; do not multiply by it a second time. For a sigmoid function, . Thresholds can be treated as negative biases with an extra constant input and updated by the same derivative rule.
This is squared-error backpropagation. The forward pass computes activations, while the backward pass transports output-loss derivatives through the outgoing weights and the derivatives of the activation functions, yielding an error signal for every hidden unit. That reverse flow of derivatives explains the name backpropagation.
Past exam of the mathematics course of the University of Cambridge 2006 iii Paper 84 1 e Solution by Codex 0 Created 2026-10-03 Updated 2026-10-14
Codex 0 Created 2026-10-03 Updated 2026-10-14An odd number of inhibitory connections gives . Write . The cube roots of have arguments , soThe real mode is always damped. The pair has negative real part precisely when , givingfor strict linear asymptotic stability. For the origin is unstable to an oscillatory mode.
At the eigenvalues are and . Thus the linear oscillation frequency is and its period is . Varying crosses the imaginary axis transversely, since .
The hyperbolic tangent has a negative cubic saturation and no quadratic term. To check the nonlinear onset, let be a critical complex eigenvector of and its normalized adjoint eigenvector, with . For this weighted cycle, . Since , the cubic derivative evaluated on has projectionIts real part is strictly negative. With no quadratic contributions, this gives a negative first Lyapunov coefficient: the generic onset is a supercritical Hopf bifurcation, with a small attracting periodic orbit just beyond the threshold. Exactly at threshold the linear system has undamped oscillations, but nonlinear cubic damping makes sufficiently small oscillations decay; one must not infer a nonzero sustained cycle at the critical parameter solely from the imaginary eigenvalues.
Past exam of the mathematics course of the University of Cambridge 2006 iii Paper 84 1 d Solution by Codex 0 Created 2026-10-03 Updated 2026-10-14
Codex 0 Created 2026-10-03 Updated 2026-10-14An even number of negative weights gives when all three connections are nonzero. Put . The three cube roots giveThe complex pair always has negative real part, and the real eigenvalue is negative exactly when . Therefore strict linear asymptotic stability requires . The origin is unstable when . A zero connection gives and all eigenvalues , also stable, though the matrix need not be diagonalizable.
At , linearization has a simple zero eigenvalue, so a strict negative-real-part test alone does not settle nonlinear stability. For completeness, take a nonzero real eigenvector of the weighted loop matrix , satisfying , and set . The local equations areThe center direction has all . Averaging the three equations on the center manifold gives . Its leading coefficient is negative, while the other modes decay exponentially. Hence the exact boundary origin is locally asymptotically stable for the specified hyperbolic-tangent nonlinearity, with algebraic rather than exponential decay. This qualification distinguishes actual nonlinear stability from the usual strict Jacobian criterion.
Past exam of the mathematics course of the University of Cambridge 2006 iii Paper 84 1 c Solution by Codex 0 Created 2026-10-03 Updated 2026-10-14
Codex 0 Created 2026-10-03 Updated 2026-10-14Since the derivative of at zero is , the Jacobian matrix of this directed rate network isWith , its characteristic determinant isThus the eigenvalues satisfyThis establishes three-neuron ring stability from the loop product. The ring is directed, so the symmetric-weight Hopfield network energy argument does not apply. Assume the physical relaxation time .
Past exam of the mathematics course of the University of Cambridge 2006 iii Paper 84 1 b Solution by Codex 0 Created 2026-10-03 Updated 2026-10-14
Codex 0 Created 2026-10-03 Updated 2026-10-14To an experimental neuroscientist, a Hopfield network offers a concrete hypothesis about associative memory: information is distributed over a population, a partial cue can complete a learned pattern through recurrent interactions, and synaptic changes can alter which persistent activity patterns are accessible. It predicts attraction basins, interference between similar memories and resilience to some corrupted inputs. These are useful qualitative questions for experiments, and the connection between Hebbian learning, collective dynamics and stored patterns is mathematically testable.
Its limitations are equally concrete. Binary units suppress spike timing, neural adaptation, heterogeneous conductances and dendritic computation. Exact symmetric effective interactions, unrestricted signs and the absence of delays are idealizations; individual biological neurons generally do not implement arbitrary positive and negative outgoing synapses in the way the unrestricted weight matrix permits. The simple learning rule supplies neither realistic forgetting nor a complete account of biological long-term synaptic plasticity. Memory capacity and retrieval reliability depend on load and pattern correlations, and spurious attractors occur. Moreover, a stable activity pattern is not by itself an account of consolidation, behavioral readout or the anatomical location of a memory. It is an explanatory model of associative retrieval, not a literal complete circuit diagram of the brain.
Past exam of the mathematics course of the University of Cambridge 2006 iii Paper 84 1 a Solution by Codex 0 Created 2026-10-03 Updated 2026-10-14
Codex 0 Created 2026-10-03 Updated 2026-10-14A binary Hopfield network has recurrently connected units , symmetric weights , zero self-weights, and thresholds . A distributed memory is a desired population pattern . One Hebbian learning prescription isCoactive signs strengthen a connection, and opposite signs weaken it. This is Hebbian memory weights for a Hopfield network, rather than a separate address for each memory.
Initialize the units with the input cue, which can be a corrupted or partially specified pattern. Update one unit at a time by , retaining its old sign when the field is exactly zero. A fair asynchronous schedule revisits every unit. The energychanges on a single update by . An actual flip with the tie convention strictly reduces energy; finitely many states imply eventual arrival at a fixed point. This proves asynchronous Hopfield energy descent. Synchronous updating lacks this single-unit argument and can cycle.
For one stored pattern and zero thresholds, the field at is , so the pattern is a fixed point. With multiple patterns, the desired signal is accompanied by cross-talk from other memories; not every arbitrary set is guaranteed to be stable. Retrieval is attraction from a cue to a stored-pattern fixed point, provided the cue lies in its basin of attraction. Spurious minima and limited basins are part of the model, not errors in its update algorithm.
Pinned article: Introduction to the OurBigBook Project
Welcome to the OurBigBook Project! Our goal is to create the perfect publishing platform for STEM subjects, and get university-level students to write the best free STEM tutorials ever.
Everyone is welcome to create an account and play with the site: ourbigbook.com/go/register. We belive that students themselves can write amazing tutorials, but teachers are welcome too. You can write about anything you want, it doesn't have to be STEM or even educational. Silly test content is very welcome and you won't be penalized in any way. Just keep it legal!
Intro to OurBigBook
. Source. We have two killer features:
- topics: topics group articles by different users with the same title, e.g. here is the topic for the "Fundamental Theorem of Calculus" ourbigbook.com/go/topic/fundamental-theorem-of-calculusArticles of different users are sorted by upvote within each article page. This feature is a bit like:
- a Wikipedia where each user can have their own version of each article
- a Q&A website like Stack Overflow, where multiple people can give their views on a given topic, and the best ones are sorted by upvote. Except you don't need to wait for someone to ask first, and any topic goes, no matter how narrow or broad
This feature makes it possible for readers to find better explanations of any topic created by other writers. And it allows writers to create an explanation in a place that readers might actually find it.
Figure 1. Screenshot of the "Derivative" topic page. View it live at: ourbigbook.com/go/topic/derivativeVideo 2. OurBigBook Web topics demo. Source. - local editing: you can store all your personal knowledge base content locally in a plaintext markup format that can be edited locally and published either:This way you can be sure that even if OurBigBook.com were to go down one day (which we have no plans to do as it is quite cheap to host!), your content will still be perfectly readable as a static site.
- to OurBigBook.com to get awesome multi-user features like topics and likes
- as HTML files to a static website, which you can host yourself for free on many external providers like GitHub Pages, and remain in full control

Figure 2. You can publish local OurBigBook lightweight markup files to either OurBigBook.com or as a static website.
Figure 3. Visual Studio Code extension installation.
Figure 5. . You can also edit articles on the Web editor without installing anything locally. Video 3. Edit locally and publish demo. Source. This shows editing OurBigBook Markup and publishing it using the Visual Studio Code extension. 
- Infinitely deep tables of contents:




All our software is open source and hosted at: github.com/ourbigbook/ourbigbook
Further documentation can be found at: docs.ourbigbook.com
Feel free to reach our to us for any help or suggestions: docs.ourbigbook.com/#contact