Lipids are a chemically diverse family of chemical substances, conventionally associated with biological origin and solubility in nonpolar solvents. They include triglycerides, phospholipids, and cholesterol. The name does not specify one molecular formula, one repeating monomer, or one kind of polymer. Some lipids have both hydrophilic and hydrophobic regions rather than being uniformly nonpolar. See IUPAC Gold Book: lipids.
Structure explains the different jobs. A triglyceride has three fatty acid-derived acyl groups attached to glycerol and serves as an energy store. A typical glycerophospholipid instead combines two such chains with a phosphate-containing head, making it an amphiphile suited to a lipid bilayer. Cholesterol has a different structure and also contributes to cell membrane properties. Thus a lipid is a chemical building material, while a lipid bilayer is an organization of many molecules. See Clark, Douglas and Choi, Biology 2e, 3.3: lipid structures and functions.
In this physiological context, a reserve or dietary material rich in triglycerides; distinct from the broader class of lipids.
The mixture of hydrophobic surface lipids, often including very-long-chain fatty-acid derivatives, that contributes to plant surface barriers.
A chemically heterogeneous plant barrier polymer with aliphatic and aromatic components, important in tissues such as roots and cork.
A plant extracellular polyester formed largely from oxygenated fatty-acid derivatives, contributing to the cuticular barrier.
A lipid class based on a steroid skeleton with a hydroxyl group; plant sterols contribute to membrane properties and biosynthetic regulation.
A lipid with a galactose-containing headgroup; galactoglycerolipids are major components of plant photosynthetic membranes.
A diacylglycerol with a digalactosyl headgroup, often abbreviated DGDG. Phosphate deprivation can increase its abundance in extraplastidial membranes.
A diacylglycerol with one galactose headgroup, often abbreviated MGDG.
lipid peroxidation oxidatively damages lipids, particularly susceptible unsaturated chains. Oxidation products can alter membrane properties and chemical stability; higher unsaturation therefore creates potential tradeoffs as well as functional opportunities.
acyl editing exchanges acyl groups between membrane-lipid and acyl-CoA pathways. Its substrate selectivity can affect flux into engineered long-chain polyunsaturated lipids.
substrate dichotomy in fatty-acid engineering describes incompatible carrier preferences of sequential reactions, especially lipid-linked desaturation followed by acyl-CoA-dependent elongation. Limited transfer between pools can block flux even when both catalysts are active.
dolichol phosphate is a phosphorylated lipid carrier used in glycan assembly. Lipid-linked sugar intermediates permit some lumenal transfer steps that do not directly use free nucleotide sugars.
dolichol is a long-chain isoprenoid lipid whose phosphorylated derivatives carry sugars or oligosaccharides during glycan assembly.
A triglyceride contains glycerol joined to three fatty acid-derived acyl groups through ester linkages. Compare the three chains with the two-chain, phosphate-headed glycerophospholipid illustrated below. See Biology 2e: fats and oils.
Cholesterol is a lipid with four fused rings and a small hydrophilic region. It helps regulate the fluidity of animal cell membranes; it is structurally distinct from a phospholipid. See Biology 2e: cholesterol.
Phospholipids are lipids containing a phosphate group as part of their structure linked by covalent bonds. The familiar membrane-forming phospholipids are amphiphilic: a hydrophilic head region with chemical polarity coexists with a hydrophobic, largely nonpolar hydrocarbon region. These descriptions refer to different parts of the same molecule, not to two separate substances. See IUPAC Gold Book: phospholipids and IUPAC Gold Book: amphiphilic.
A typical two-chain glycerophospholipid provides a useful example: a glycerol scaffold carries two fatty acid-derived acyl groups through ester linkages, plus a phosphate-containing head region. Phosphatidylcholine is one example. This scaffold describes an important subclass, rather than all phospholipids: sphingomyelin has a different backbone, and even glycerophospholipids need not all have two acyl groups. See IUPAC–IUB, Nomenclature of Lipids (1976), Lip-1.5 and Lip-2.1–2.6.
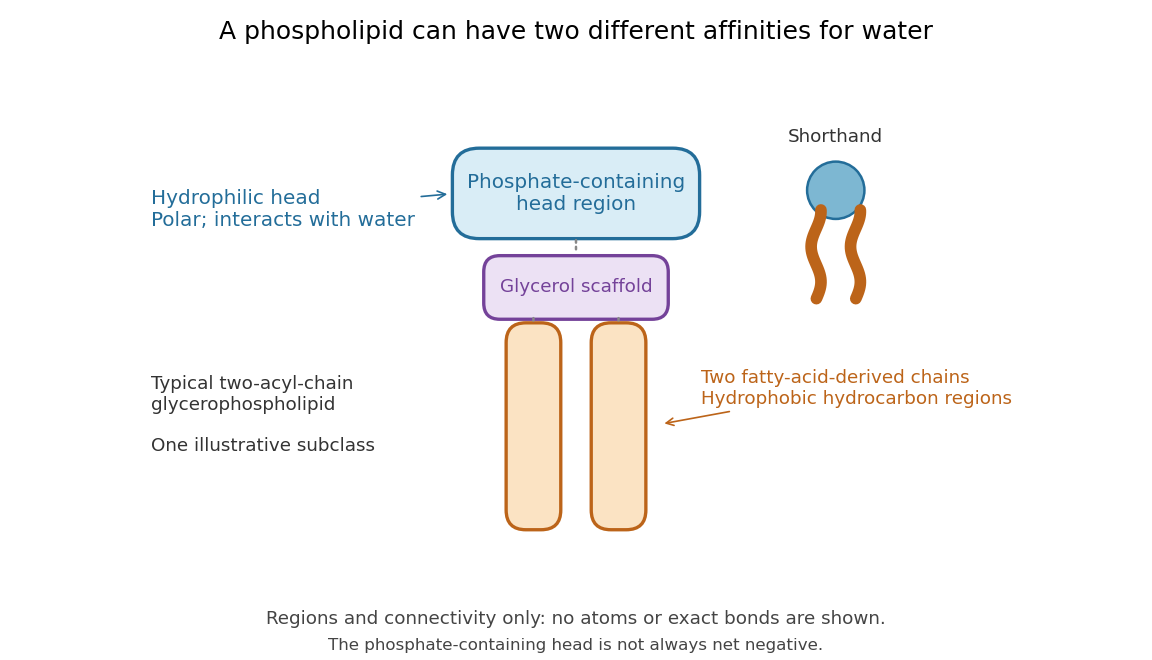

Polar does not mean negatively charged overall. At near-neutral pH, phosphatidylcholine is zwitterionic: its phosphate region carries negative electric charge and its choline region positive electric charge, with zero net electric charge for the molecule. Counting those opposite charges gives ; it does not remove their local interactions with water. See Lodish et al., Molecular Cell Biology: membrane lipids.
In a lipid bilayer, two membrane leaflets orient their hydrophilic heads toward the water on either side and their hydrophobic chains toward the shared interior. The hydrophobic effect helps explain this organization through the free energy of the water and lipids together. It is not a special repulsive chemical bond between chains and water. Which organization is favored also depends on molecular geometry, temperature, concentration, and the surrounding chemical solution; a phospholipid label alone does not guarantee a lipid bilayer. See Alberts et al., Molecular Biology of the Cell: the lipid bilayer.
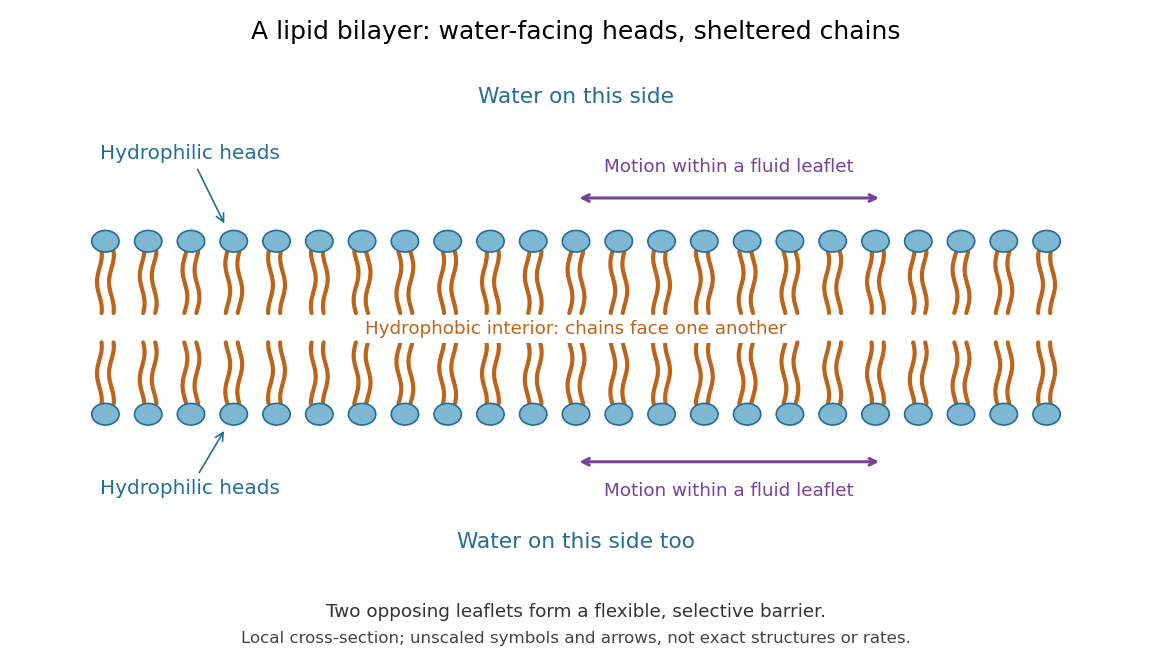

This organization supplies a flexible barrier for compartments. A fluid lipid bilayer allows lipids to undergo diffusion within each membrane leaflet; barrier function therefore coexists with motion of molecules, as in the fluid mosaic model. It is not completely impermeable: small nonpolar molecules such as molecular oxygen and carbon dioxide cross much more readily than ions. In a cell membrane, ion channels and other membrane transport proteins provide selective routes; the existing membrane transport article explains their driving forces. See Alberts et al.: principles of membrane transport.
In 1925, E. Gorter and F. Grendel extracted lipids from red blood cells and compared the surface area of a one-molecule-thick film on water with the estimated total surface area of the red blood cells. Their table gave ratios near two, supporting a two-layer covering; they also proposed heads facing the aqueous surroundings on both sides. The inference depends on recovering the relevant lipids, estimating the red blood cell surface area correctly, and comparing compatible packing in the film and the cell membrane. It was indirect evidence, not an image of the lipid bilayer. The paper itself notes possible losses during evaporation. See Gorter and Grendel, On Bimolecular Layers of Lipoids on the Chromocytes of the Blood, Journal of Experimental Medicine 41 (1925), 439–443.
phosphatidylinositol is a glycerophospholipid with an inositol headgroup. phosphorylation of that headgroup produces distinct phosphoinositides.
A phosphoinositide is a phosphorylated derivative of phosphatidylinositol. Phosphate position changes the recognition surface of the headgroup, allowing distinct species to recruit different membrane-associated proteins.
A phosphoinositide enriched in particular membrane domains, including Golgi-associated compartments.
phosphatidylinositol 3,5-bisphosphate is a doubly phosphorylated phosphoinositide involved in later endolysosomal organization and function. Perturbing it need not imply that initial surface uptake is defective.
phosphatidylinositol 3-phosphate is a phosphoinositide associated with endosomal membrane identity and recruitment of specific effectors.
phosphatidylinositol 3,4-bisphosphate has phosphates at positions 3 and 4 of the inositol ring. Local production can contribute to timed recruitment of endocytic membrane-remodeling factors.
A lysophospholipid is a phospholipid derivative missing an acyl chain relative to its corresponding diacyl form. The changed headgroup-to-tail geometry can alter curvature preference and bilayer stability.
Glycerophospholipids are phospholipids built on a glycerol-phosphate scaffold. The illustrated two-acyl group form is common, but the subclass also includes other substitutions and one-chain derivatives. See IUPAC–IUB lipid nomenclature, Lip-2.2 and Lip-2.6.
phosphatidylserine is a glycerophospholipid with a serine-containing headgroup that is normally net negatively charged near physiological pH. Its leaflet distribution contributes to membrane surface properties and protein recruitment.
phosphatidylethanolamine is a glycerophospholipid with an ethanolamine headgroup. Its relatively small headgroup can favor negative monolayer spontaneous curvature, depending on chain composition and conditions.
Phosphatidylcholine, abbreviated PC, is a glycerophospholipid with a phosphate-choline head. Its zwitterionic head illustrates why a hydrophilic region need not have a nonzero net electric charge. See Lodish et al.: membrane lipids.
Sphingomyelin is a phospholipid whose backbone is based on sphingosine, rather than glycerol. One long hydrocarbon region belongs to that backbone and another comes from an attached fatty acid. It is a counterexample to defining every phospholipid by the illustrated glycerol scaffold. See Cooper, The Cell: the molecular composition of cells.
Articles by others on the same topic
There are currently no matching articles.