This University of Oxford Part B paper covers Mathematical Ecology and Biology in section A and Nonlinear Systems in section B. It is cross-listed for Mathematics, Mathematics and Computer Science, and Mathematics and Statistics. [ref]
https://www.whatdotheyknow.com/request/maths_past_papers_3. Source release
A bounded official-source search found no advertised answers for this exact paper. The complete archive transcription retains its supplied graph and printed map; the solutions include the antipodal two-cycle lost by the proposed quadratic reduction.For the Ricker population map , fixed points satisfy or . Thus zero exists for all , while is positive exactly when . Since , the respective periodic-orbit multipliers are and .
Consequently zero is linearly attracting for and repelling for ; the positive biological population is linearly attracting for and repelling for . The periodic-orbit multiplier of the positive point is positive below and negative above it, distinguishing monotone from alternating local convergence. At , the coincident zero state has unit periodic-orbit multiplier but for every , giving nonlinear attraction from the physical right side. At the periodic-orbit multiplier is and linearization is inconclusive. Writing , the second iterate has expansion , so the critical point is weakly attracting; beyond it a period-doubling instability occurs.
A large initial biological population maps to a very small positive biological population because at large : the initial slump is followed by recovery. Cobwebbing alternates a vertical step from to with a horizontal step to the diagonal at . The figure uses the explicit illustrative choice .
For , every positive orbit subsequently lies below the maximum . On the map is increasing, with the unique positive fixed point . Below that point and ; above it and . Therefore the trapped iterates approach the fixed point monotonically from whichever side they enter. In particularThe extinction initial value remains zero, but exact extinction is never reached from a positive finite biological population in this deterministic model.
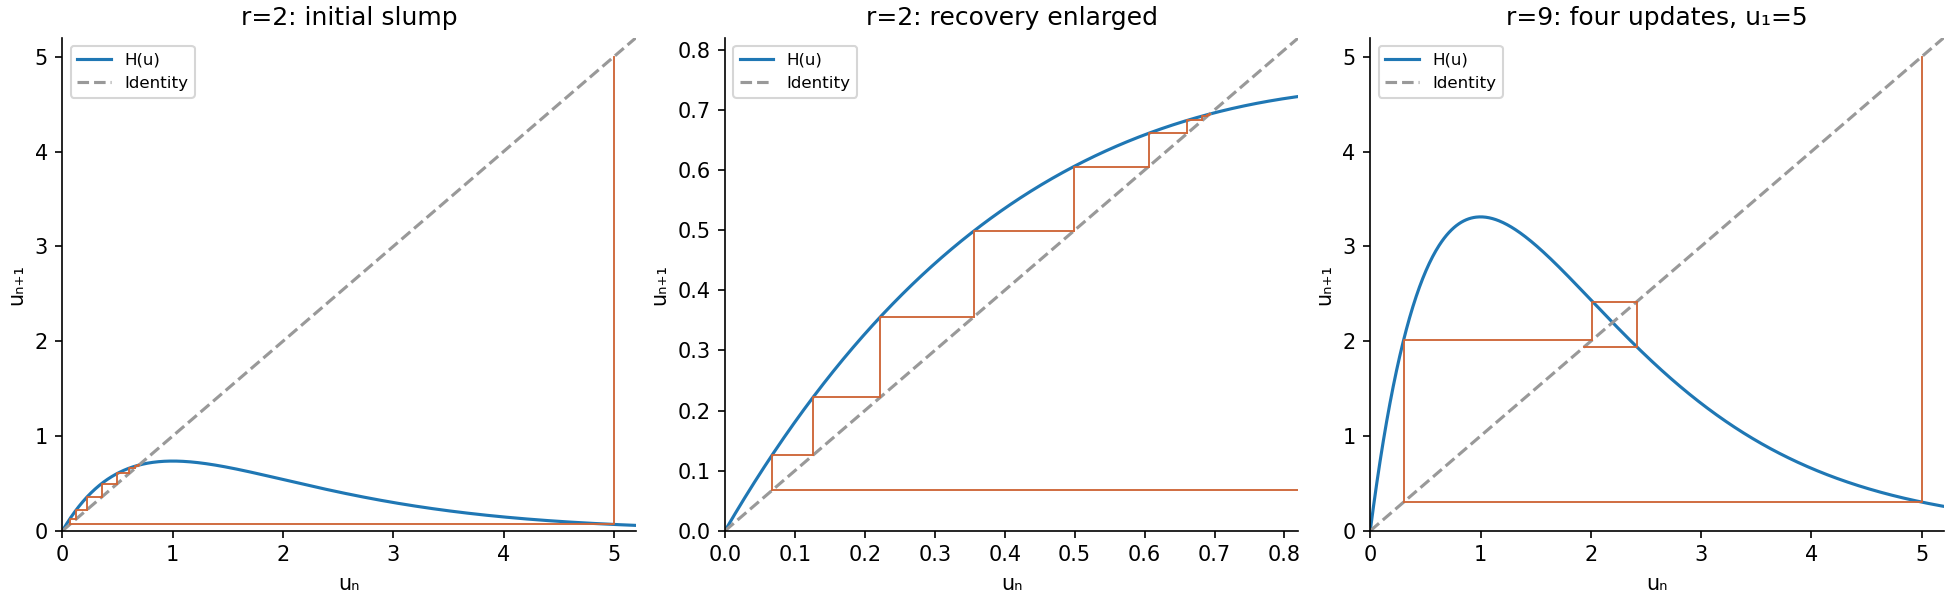
Apply the same vertical-then-horizontal cobweb construction to . Since no numerical value of the large initial biological population is prescribed, an exact five-generation list is , , , , . For the plotted example , these values areThe initial slump is followed by rapid growth and an alternating overshoot about , which is now unstable because its periodic-orbit multiplier . A still larger initial biological population can remain extremely small for more than these four updates; the example illustrates the requested construction without imposing an unstated universal numerical starting value.
For , the second-iterate equation is equivalent to . Write and let paired points be . The condition becomes . At , , so strict concavity of the positive hyperbolic tangent gives one nonzero positive , as well as . Here it is exactly .
Thus the four nonnegative fixed points of areZero has periodic-orbit multiplier and the central point has periodic-orbit multiplier , so both are unstable. The outer two points are exchanged by , since and . Their common second-iterate periodic-orbit multiplier isIts magnitude is below one, so both outer fixed points of are stable. This verifies the crossings and stability in the supplied graph rather than reading stability from crossing direction alone.
The Ricker population map two-cycle consists of the two stable points of the second iterate, exchanged by the original map. Thus generic positive orbits approach alternating valuesThere are exceptions: zero stays extinct, while an orbit starting at or at one of its finite preimages eventually stays at that unstable fixed point.
To justify the large-time conclusion, put and . Every first image is at most . A positive orbit below grows until it enters ; if it never entered, its monotone limit below would contradict the fixed-point equation. The interval is invariant. On it is decreasing, so is increasing. Its only fixed points there are the three positive points already found; its graph signs make iterations below the unstable middle point converge to the lower stable point, and those above converge to the upper stable point. Interchanging even and odd subsequences under then gives the stated two-cycle. This is regular period-two behaviour, not chaos at this parameter.
Let . The given expansion implies and thereforeUsing gives preciselyThe paired low value is . It is small, so andBy the chain rule the second-iterate periodic-orbit multiplier is their product:Since while , this tends to and eventually has magnitude above one. Thus the large second-iterate fixed point, and hence its associated two-cycle, is unstable for sufficiently large . The high state's small derivative alone does not imply stability: the low state's derivative supplies the compensating factor of order .
The law of mass action assigns infection rate , death rate , and vaccination rate . Vaccination consumes a susceptible animal and produces a vaccinated one while leaving the triggering infected animal present. In dimensional time ,All compartment counts remain nonnegative. Adding the equations gives ; deaths are retained in the bookkeeping compartment rather than removed from that conserved count. There is no recovery class of live immune survivors in the infection reaction: in this particular model every animal that becomes infected ultimately dies.
Use and scale each count by the susceptible infection threshold :For example , while . Dividing all equations by therefore givesThus measures the vaccination response relative to transmission in this mass-action model. The total dimensionless count is conserved, and the instantaneous infection growth threshold is .
While and , division of the equations gives and . Integrating from the initial data yieldsLet be the final susceptible level. Using givesThis is the smaller positive root selected by decreasing susceptibility; the function is decreasing on , so that selected root is unique. Its upper bound below also follows directly because the added positive term moves the decreasing-branch root left.
Conservation of the total count, or integration of , then gives the number killed, including those initially infected:The remaining susceptible loss is split between infection and vaccination in fixed ratio ; this explains the factor multiplying .
Rearrange the final-size equation as . With fixed and , the selected root is exponentially small:Substitution into the death count yieldsThus strong vaccination suppresses most secondary fatal infections but cannot save the animals already infected, as required by the stated reaction scheme. The limit holds for the fixed positive initial infection assumed here; it need not be uniform if is allowed to shrink with increasing .
For the vaccinated epidemic-wave final size, write . From the travelling-wave equations, and . Using the ahead-of-wave boundary data givesAdding the four wave equations yields . Integrate once and use to obtain . At minus infinity the assumptions therefore give .
Combining these identities shows that satisfiesThe nontrivial positive epidemic-wave root has ; the other root is the disease-free solution. The assumed positive wave consequently requires ; for the displayed relation has no distinct smaller root.
At the back of the pulse there are no infectives, so the live biological population consists of susceptible and vaccinated animals:The final-size root is independent of vaccination strength in this travelling-wave problem; vaccination instead changes the split between deaths and survivors for the total biological population lost from susceptibility.
From the preceding conservation identity,The nontrivial root depends only on , through . Therefore the coefficient is independent of , proving the exact requested proportionality to , conditional on existence of the positive wave. This is stronger than an asymptotic estimate and differs from the spatially homogeneous problem with a fixed positive initially infected count.
Set , and . Then and , givingThe common carrying-capacity scale becomes one, while is the ratio of the two intrinsic growth rates. Intraspecific competition is twice as strong as the cross-species effect in these dimensionless equations.
In coordinate order the Jacobian matrix isAt the origin it is , giving a repelling node equilibrium; when the repeated positive eigenvalue is semisimple. At coexistence it isIts trace is , determinant , and characteristic discriminant . Hence both eigenvalues are real and negative, proving a stable node equilibrium for every .
The other equilibria are and . Their triangular Jacobians have eigenvalues and respectively. Thus both single-species equilibria are saddles, with their attracting directions on the corresponding coordinate axes and unstable directions allowing invasion by the other species. There are no further nonnegative equilibria because the two non-axis nullclines intersect only at .
The non-axis nullclines are and , intersecting at . Each biological population grows below its own line and decreases above it. The axes are invariant; along a positive axis the surviving species follows logistic growth towards its unit carrying capacity. The origin remains fixed.
All strictly positive initial states converge to coexistence. An entropy-shaped Lyapunov function for weak competition proves the global conclusion beyond the local arrows: put and useEach bracket is nonnegative, vanishing only at its equilibrium value, and tends to infinity at zero or infinity. Differentiation givesThus positive trajectories remain in a compact level set inside the quadrant and approach its unique zero-derivative state. ThereforeThe phase portrait shows the stable coexistence point, invading directions near the axis saddles, and the two straight nullclines.
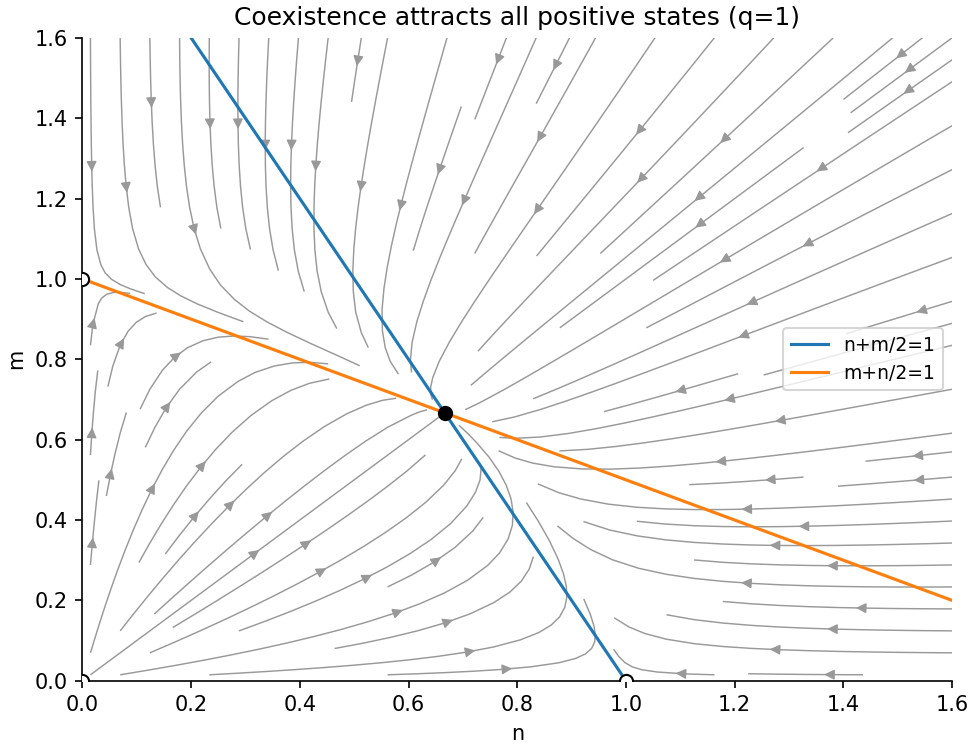
Competing populations converge to coexistence in the positive quadrant
. Details. The coexistence Jacobian matrix calculated in part (a) has negative diagonal entries and positive determinant. For any spatial mode with squared wave number , the linearized matrix is . Its trace is more negative than before, and its determinant isHence both eigenvalues retain negative real parts for every mode and every . This is the mechanism by which negative self-response excludes two-species Turing instability, excluding diffusion-driven instability using only the reaction Jacobian matrix already computed, together with the diagonal diffusive damping. In particular unequal diffusion is not enough to produce a Turing pattern when both local self-responses are negative in this two-species competitive model.
For , has eigenvectors and with eigenvalues and . The Neumann spatial modes are , . Combining each with those two reaction directions gives temporal ratesEvery linear perturbation therefore decays at least as fast as . The slowest mode is the spatially uniform antisymmetric change of the two biological populations. ThusSmall nonlinear perturbations have the same bound, not just a formal mode calculation. In one spatial dimension take sufficiently small smooth Neumann data, or small data in a norm such as that controls quadratic products. The linear semigroup decays at rate , and the nonlinear remainder is quadratic. Standard small-data variation-of-constants estimates first give decay for any fixed . Choose ; then the remainder is , and its Duhamel convolution with is because . This sharpens the preliminary bound to the displayed rate. Special initial data with no slow-mode component may decay faster, but the general estimate cannot be improved uniformly.
An equilibrium is asymptotically stable when it is Lyapunov stable and attracts every initial state in some neighbourhood. Lyapunov stability means that sufficiently small initial displacement stays small for all future times; attraction additionally requires convergence to the equilibrium. A Lyapunov function is a differentiable positive-definite scalar function near the equilibrium whose derivative along solutions is nonpositive. Strict negativity, or an appropriate invariant-set argument for a non-strict derivative, gives asymptotic stability.
For , equilibria satisfy and , so only is real. Its Jacobian matrix is , with eigenvalues for every . It is a linear centre equilibrium, so linearization alone cannot decide nonlinear attraction.
Use the positive proper energyFor , energy sublevel sets are compact and invariant. The zero-derivative set is the union of the axes, but its only invariant subset is the origin: on one immediately leaves that axis, and on one has . LaSalle's invariance principle therefore proves global asymptotic stability. At the conserved energy levels are closed periodic orbits, giving a nonlinear centre equilibrium. For , time reversal together with converts the system to the attracting negative- case, so the origin is a nonlinear repeller and is unstable. Nonzero forward trajectories cannot remain bounded; this does not assert existence for all time if finite-time escape occurs.
At either nonzero point the Jacobian matrix is , with eigenvaluesBoth points are attracting for and repelling for . For they are stable foci; for stable nodes. For they are unstable foci; for unstable nodes. At the two repeated-root boundaries they are degenerate nodes. At , linearization has purely imaginary eigenvalues; the conserved energy in the next part shows that they are actual nonlinear centres. Thus the zero-real-part case is resolved by an additional first integral, rather than by the linear test alone.
For , the first integral isIts minimum occurs at the two centres. Levels between and give a periodic orbit around each centre equilibrium; positive levels give larger periodic orbits surrounding both wells. The zero level is the figure-eight separatrix through the saddle, with two homoclinic loops.
On , . The printed parametrization , , taking matching signs, satisfies this identity because . It also has and , so its parameter is physical reversed time, , rather than . It is nonetheless exactly a parametrization of the requested trajectory. In physical forward time one can use , on the right loop.
Approach to the origin requires , hence infinite physical time. Equivalently near the right-loop endpoint, so the elapsed time contains the divergent integral . The point at is reached in finite time from any interior point; it is the asymptotic saddle endpoints, not that turning point, that cause the infinite total traversal time.
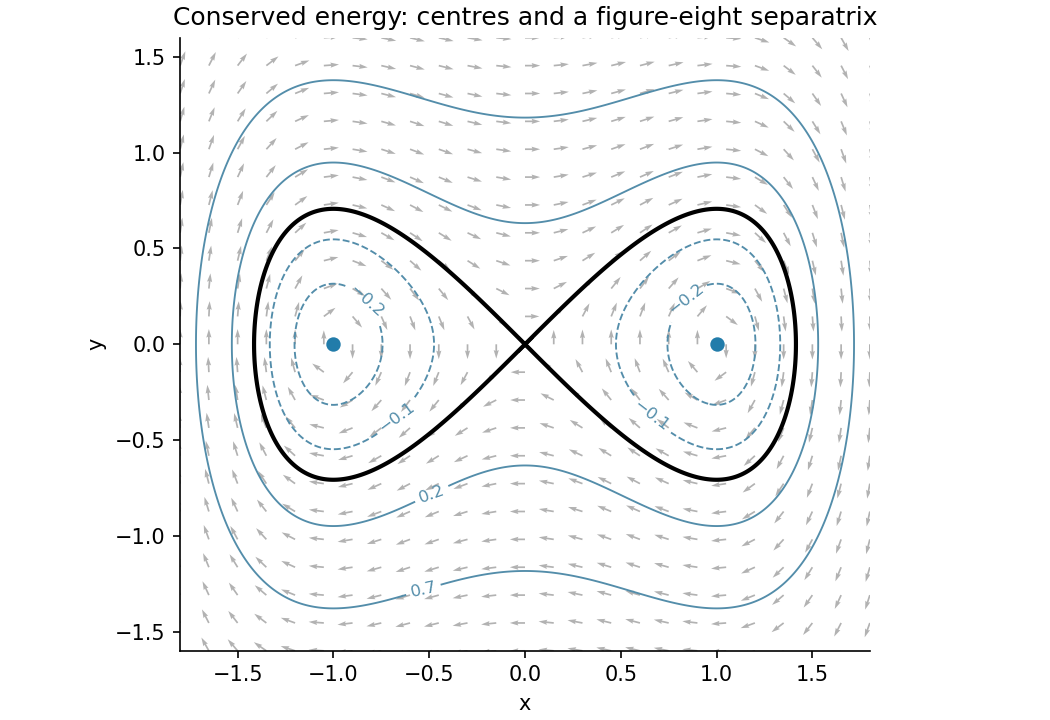
Double-well energy levels and the two homoclinic loops through the saddle
. Details. The cubic terms vanish in the linearization, leaving . Its eigenvalues are , so the origin is a repelling focus equilibrium. The nonzero imaginary part gives rotation, while the positive real part makes small amplitudes grow. In particular it cannot be the forward limit of nearby nonzero trajectories, which motivates looking for an attracting periodic orbit away from the origin.
Use , with . Dotting the vector field with the radial direction and taking its angular cross-product givesThe angular factor ranges from one to three. Hence every radial component is outward for , and every radial component is inward for . The limiting radii areThere is a minor strictness point in the wording. At the outward inequality is non-strict, with tangencies where ; at the inward inequality is non-strict, with tangencies where . Thus these are the supremum and infimum for strict crossing at all angles. The weak inequalities at the endpoints are exactly what is needed for the closed trapping annulus in the next part.
The closed annulus is positively invariant by the radial signs, and excludes equilibria there. Poincaré-Bendixson therefore yields a periodic orbit. Its stability can be established explicitly rather than inferred merely from trapping.
For the exact anisotropic radial limit cycle, set . Then , or . Its unique periodic solution isIt is positive and stays within the trapping annulus. Any other solution at the same phase has , proving radial attraction and uniqueness of the positive periodic orbit. The full planar period is , since a full angular revolution takes that time; the half-turn symmetry of the radius does not halve the period of the position vector. The nontrivial return periodic-orbit multiplier is . Thus the periodic orbit is asymptotically stable, and all nonzero forward trajectories approach it up to phase.
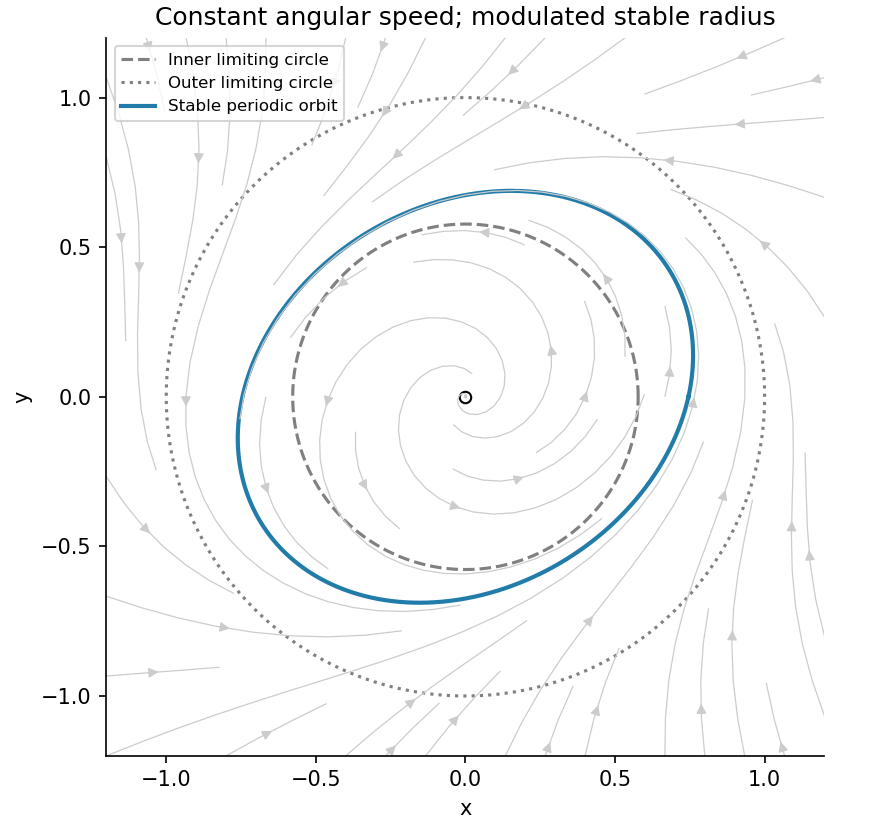
The trapping annulus and the explicitly attracting angularly modulated limit cycle
. Details. A fixed point of a map satisfies . Its linear perturbations evolve by the Jacobian matrix : both eigenvalues must lie strictly inside the unit disk for linear asymptotic stability. One inside and one outside gives a saddle; both outside give a repeller. Unit-modulus eigenvalues require nonlinear analysis, unlike the continuous-time test using signs of real parts.
Here a fixed point has and . ThereforeAt zero the characteristic equation is . Its negative root is less than for every , while its positive root crosses at . Thus zero is a saddle for and a real repeller for , with a pitchfork of fixed-point branches at .
At either nonzero point the characteristic equation is , whose discriminant is . For the fixed points are saddles. At their periodic-orbit multipliers are , giving a flip threshold. For they are attracting real nodes; at repeated-eigenvalue degenerate nodes; and for attracting foci. The Jury stability criterion conditions reduce to and , confirming the full stable interval.
At the periodic-orbit multipliers are . For larger they form a repelling focus equilibrium. This is a unit-circle crossing at a strong resonance of a planar map with ratio ; linearization alone does not justify asserting a generic nonresonant Neimark-Sacker bifurcation. The period-two branch at the flip threshold is derived next, including an additional family absent from the source's proposed quadratic.
A genuine two-cycle must have the form with . Hence . Subtracting givesLet and . Using in either original equation gives . The cubic swap-map two-cycle factorization exhibits two cases, so cancellation of would lose an actual branch.
If , then and . Thus the source's quadratic holds for this family, withThere are two reflected genuine cycles for , coalescing with the fixed points at . For their two-step Jacobian matrix, and . The unit-disk necessary inequality fails, since it is . Therefore these quadratic-family cycles are unstable for every . For these unstable asymmetric cycles of a cubic swap map, their periodic-orbit multipliers are real: one exceeds , while the other crosses at . They are saddles before that secondary threshold and repelling beyond it. Their presence on the stable side of the fixed-point flip identifies the unstable branch of a subcritical flip.
If , then and the preceding quadratic identity gives . Hence there is also the exact cycleThis antipodal cycle of a cubic swap map does not satisfy the printed condition: its product is . Along it the one-step Jacobian matrix is the same matrix at both points, so the cycle periodic-orbit multipliers are the squares of the roots of . The Jury stability criterion conditions giveAt its periodic-orbit multipliers are on the unit circle and linearization is inconclusive. Its real-to-complex transition occurs at . Thus the printed assertion about all period-two components is incomplete: it describes only , whereas the omitted antipodal cycle supplies the actual stable period-two interval.
The fixed-point branches are and beginning at . Zero is a saddle before that threshold and repelling afterwards. The nonzero branches are saddles until , attracting for , and repelling beyond their resonant unit-circle crossing. Solid portions in the diagram mark attracting states; dashed portions mark saddles or repellers.
At , the two asymmetric two-cycles split from with components , pairing the two values with the same first sign. These branches are always unstable. In addition, the antipodal two-cycle occupies the constant component levels for every , attracting only below . It must be included for the actual printed map, even though the quadratic proposed in the previous part misses it. At a given parameter the two component levels represent one cycle, rather than two independent fixed points.
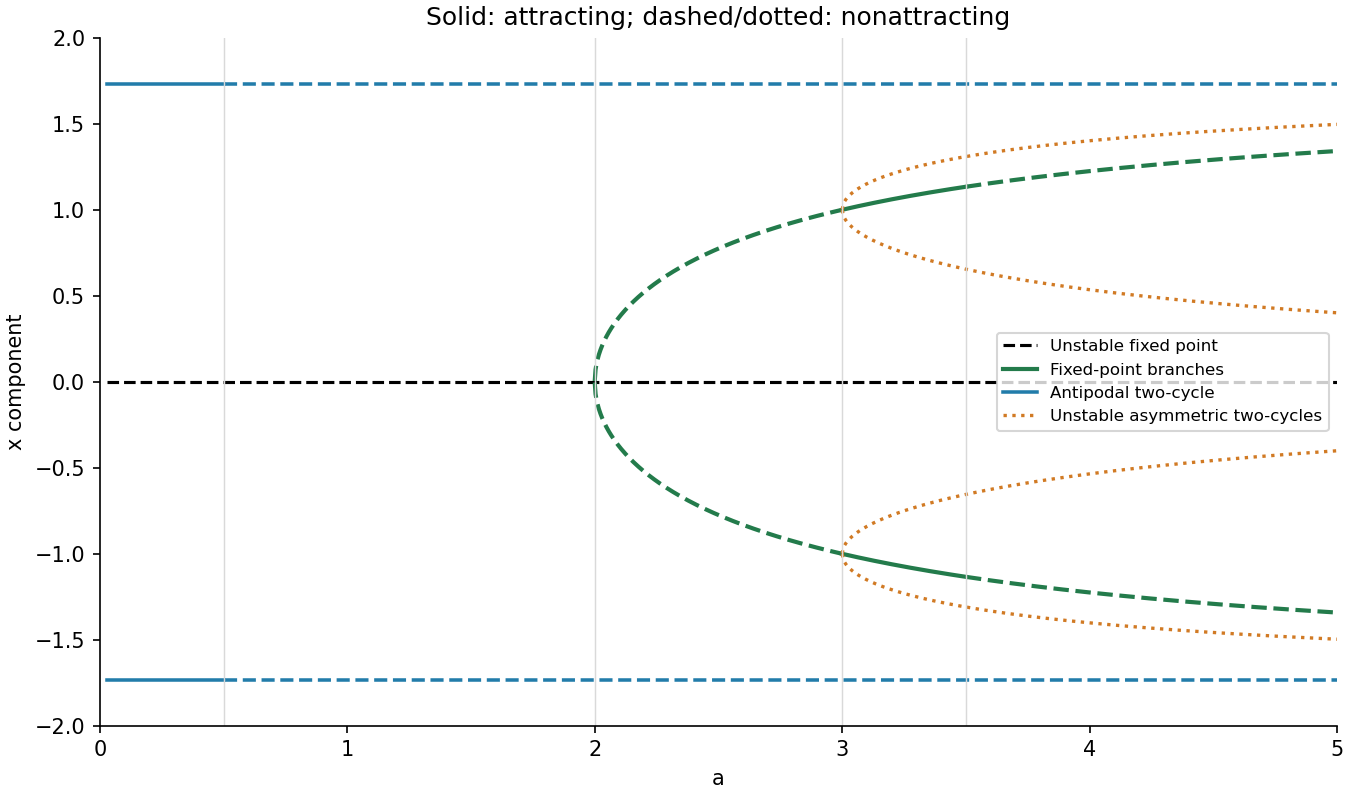
Fixed-point branches and both families of period-two cycles for the printed two-dimensional map
. Details. For an equilibrium at zero, the local stable manifold consists of nearby points whose forward trajectories remain nearby and tend to zero; the local unstable manifold is defined by backward trajectories with the analogous property. For a smooth system with , and no zero-real-part eigenvalues, the stable-manifold theorem gives manifolds tangent to the negative- and positive-real-part eigenspaces. Their dimensions are the corresponding eigenvalue counts. Real distinct eigenvalues alone are insufficient if one is zero; then a centre equilibrium direction requires additional analysis. In the saddle case each manifold is a curve, found by imposing invariance on a power-series graph through the relevant eigenvector.
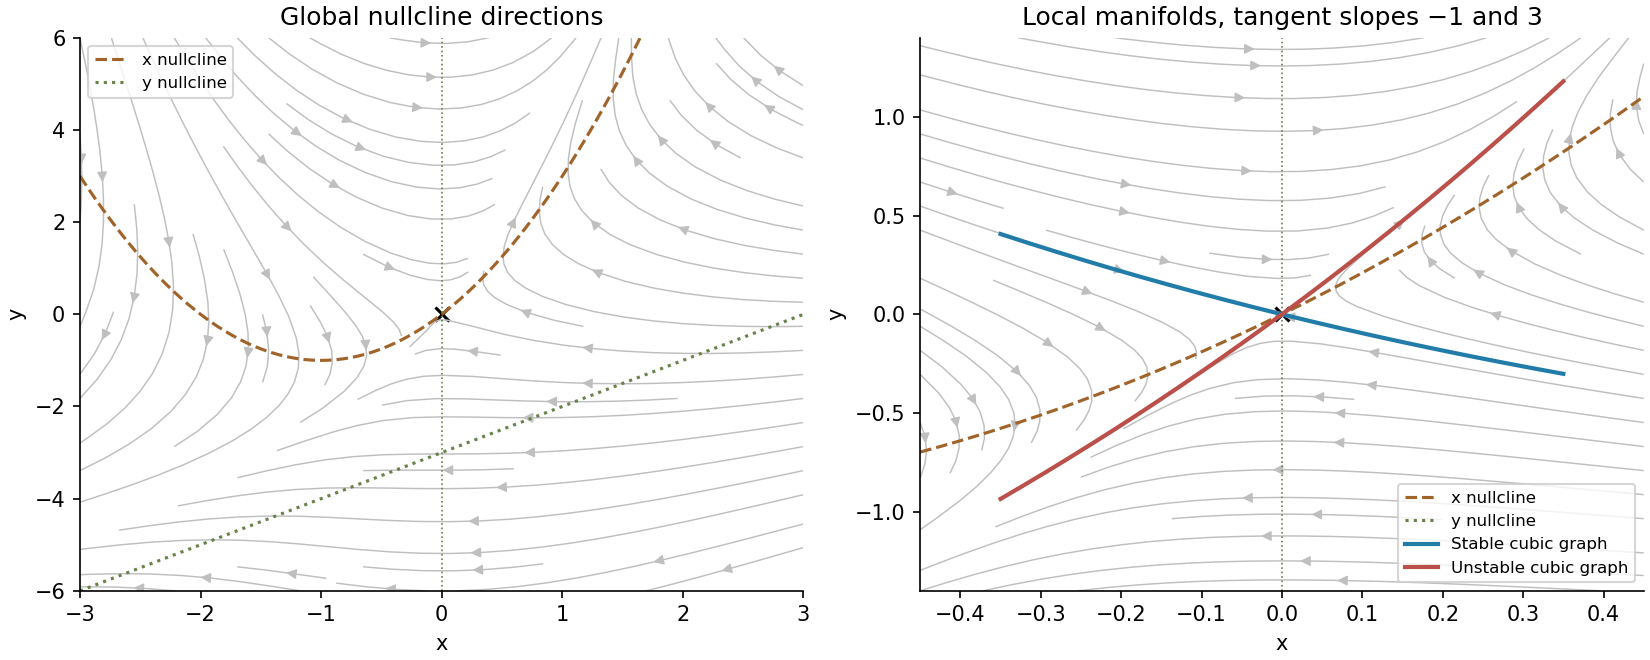
In this system, the nullcline is and the nullclines are and . Substituting the first into the second gives . Since the quadratic has discriminant , the origin is the only real equilibrium. Its Jacobian matrix has eigenvalues , with eigenvectors and . It is therefore a hyperbolic saddle.
Set for either manifold. Invariance requiresFor , matching the linear coefficient gives or . The quadratic and cubic coefficients respectively satisfyFor the stable slope , this yields , ; for the unstable slope , it gives , . ThusSubstituting back into gives the reduced dynamicsThe signs of the linear terms confirm attraction and repulsion along the respective curves.
In the phase portrait, is positive above its parabolic nullcline and negative below it; has sign . The stable branches approach the saddle and the unstable branches leave it in opposite directions. There can be no periodic orbit, since such an orbit would require total enclosed equilibrium index , while the only equilibrium has index . There is no homoclinic excursion either: eliminating gives , so a positive turning point is a strict local minimum and a negative one a strict local maximum. A loop returning to zero would require the opposite extremum somewhere. Hence bounded forward trajectories lie on the stable manifold and approach zero; other trajectories eventually leave compact regions, without a claimed universal rate or infinite-time existence at infinity. The figure shows the global nullclines and the local cubic manifold approximations; the latter are used only near zero.


Articles by others on the same topic
There are currently no matching articles.