Topics (384k) Articles (398k) Users (410) Discussions (242) Comments (383) Files (13k) New article
Biology 2e by Mary Ann Clark and others 8.1 Overview of Photosynthesis by  Codex 0 Created 2026-10-18 Updated 2026-10-31
Section of Biology 2e by Mary Ann Clark and others. Whole-book authors: Mary Ann Clark, Matthew Douglas and Jung Choi; no separate section byline is established. OpenStax publishes and hosts the text. The book was published on 28 March 2018; no separate section revision date is established.
Inspected locators: Basic Photosynthetic Structures, Figure 8.6; The Two Parts of Photosynthesis, Figure 8.7; citation information.
Biographical Memoirs: Volume 73 Carl David Anderson by William Hayward Pickering by Codex 0 2026-10-18
Codex 0 2026-10-18By William Hayward Pickering, credited as William H. Pickering. Memoir pp. 24–38; institutional issuer: National Academy of Sciences.
In the aqueous model here, a strong base supplies hydroxide essentially completely under the conditions considered. Strength and concentration are different properties.
A small single-stranded-DNA bacteriophage used in molecular-genetics research. Its compact genome made it useful for testing relationships among sequence, genetic organization and viral function.
In 1997, Hiroyuki Noji and colleagues attached a fluorescent actin filament to the central shaft of isolated . With ATP supplied, the marker made sustained rotations. This exposed rotation directly, but used ATP hydrolysis: there was no membrane motor producing ATP from a proton-motive force in this assay.[ref]
Direct observation of the rotation of F1-ATPase by Hiroyuki Noji and others. Noji, Yasuda, Yoshida and Kinosita Jr., Direct observation of the rotation of F1-ATPase, Nature 386 (1997), 299–302, accessible primary abstract
A subsequent primary experiment made the optical readout much faster. Purified Escherichia coli was immobilized on glass in a -deep flow cell, with a gold bead attached to . With ATP and magnesium supplied, laser illumination and dark-field microscopy recorded bead positions at or frames per second. The position trajectory resolved turns and intervening dwells. This apparatus follows a shaft-attached marker, rather than imaging the shaft's chemical atoms.[ref]
Temperature Dependence of Single Molecule Rotation of the Escherichia coli ATP Synthase F1 Sector Reveals the Importance of γ-β Subunit Interactions in the Catalytic Dwell by Mizuki Sekiya and others. Sekiya et al., 2009, Experimental Procedures: Direct Observation of gamma Subunit Rotation; Results, Figure 1
Controls addressed perturbation and chemical activity: comparison of – probes found similar rates for the two smallest sizes, supporting low drag; a separate coupled-enzyme assay followed ATP hydrolysis through NADH absorbance. But the rotational analysis excluded pauses longer than , so it characterizes continuously active intervals, not total output including long inhibited periods. It neither counts transported protons nor measures simultaneous single-molecule ATP synthesis.[ref]
Temperature Dependence of Single Molecule Rotation of the Escherichia coli ATP Synthase F1 Sector Reveals the Importance of γ-β Subunit Interactions in the Catalytic Dwell by Mizuki Sekiya and others. Sekiya et al., 2009, Experimental Procedures: Assay methods and data selection; Results: Direct Observation of Rotation Using a 60-nm Gold Bead
The experimental distinction is essential. Sustained directional marker motion tests a rotary mechanism. Demonstrating proton-driven synthesis additionally requires intact in a membrane with a controlled proton-motive force and a chemical ATP-production readout; dependence on that driving force and inhibition or respiratory uncoupling controls then test the proposed energy coupling. A rotation movie alone cannot establish the complete material and free energy ledger.
Define side as the higher proton electrochemical potential reservoir and side as the synthesis-side reservoir. For transfer at common temperature , define the positive downhill proton-motive force magnitude byHere is thermodynamic activity, is electric potential, is the molar gas constant and is the Faraday constant. Thus both a higher proton thermodynamic activity and a more positive electric potential on side contribute to the driving magnitude. This definition fixes the sign; conventions for a signed proton-motive force differ. The calculation under chemiosmosis separates these two contributions numerically.
Assume fixed reservoirs, tight mechanical energy coupling, one transported proton per subunit per revolution, and three ATP produced per revolution. Neglect leaks, slipping and membrane transport of the chemical reagents. Let be the local molar Gibbs free energy cost of ATP formation at the stipulated composition, pH and magnesium-binding convention. It is not necessarily the standard state value. Adding changes in the state function gives, per mole of complete turns,For this model net synthesis is thermodynamically favoured when . Equality is a reversible balance, not a promise of a useful reaction rate. A negative value establishes an available driving margin; it does not specify how fast the enzyme runs.
Choose , , and . These are illustrative inputs, not measurements of the preparation in the experiment below. Thenand . Per ATP, the ideal input is , leaving a driving margin of . The balance point isAt the same synthesis cycle instead has : the chosen reservoirs favour its reverse.
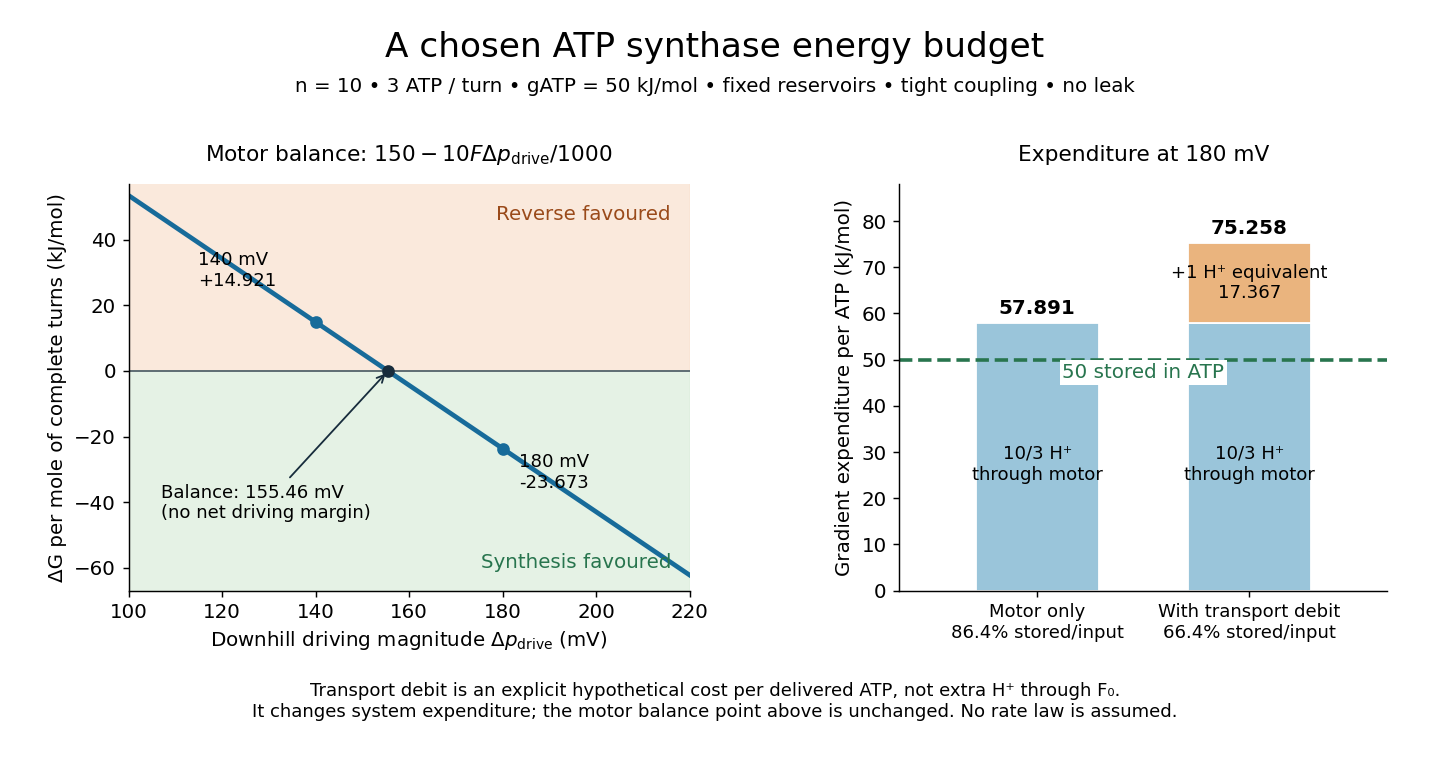
The machine is reversible: sufficient ATP hydrolysis can drive opposite rotation and pump protons uphill. Actual direction also depends on inhibition and available substrates; a weak proton-motive force need not make every intact enzyme immediately run backward. Respiratory uncoupling supplies a different failure mode: a parallel proton leak dissipates the gradient without productive shaft rotation.[ref]
Rotary catalysis of FoF1-ATP synthase by Rikiya Watanabe. Watanabe, 2013, p. 51 and Figure 2: reversal of the coupled motors
The motor budget is not the whole cost of ATP delivered outside a mitochondrion. Import of ADP and inorganic phosphate, and export of ATP, also draw on the electrochemical gradient.[ref]
The Mechanism of Oxidative Phosphorylation. Cooper, The Cell: A Molecular Approach, 2nd edition, Transport of Metabolites across the Inner Membrane, Figure 10.12
For a deliberately simplified system budget, assign these transports together one additional downhill-proton equivalent per delivered ATP, valued at the same . This is a chosen accounting convention, not a claim of one extra literal proton through , nor a universal transport stoichiometry. The total becomes equivalents and of gradient expenditure per delivered ATP at . The ratio of stored chemical free energy to that expenditure is , compared with for the motor alone. This system budget changes the resource expenditure, not the motor's balance point . Real transport terms require their own electrochemical potentials, and leaks add further cost.The membrane motor contains a rotating ring of subunits beside stationary subunit . Two offset water-accessible half-channels connect opposite membrane sides to the ring. A proton enters one half-channel and protonates a glutamic acid residue on a subunit; neutralization permits that site to enter the hydrophobic lipid bilayer. Rotation carries it around to the other half-channel, where it releases the proton. A conserved arginine in subunit helps separate the routes and promotes release. Downhill proton transfer biases rotation; this is not a freely open transmembrane pore.[ref]
Structure of a bacterial ATP synthase by Hui Guo and others. Guo, Suzuki and Rubinstein, Structure of a bacterial ATP synthase, 2019, Figure 4B–D and Proton translocation through the FO region
The central shaft transmits torque to ; a peripheral stalk prevents the catalytic head from simply co-rotating. Its three catalytic sites, within an head, cycle through different binding shapes. In the simplified binding-change picture, a loose site captures ADP and inorganic phosphate, a tight site favours bound ATP, and opening releases ATP. Rotation changes binding and release as well as chemistry.[ref]
Structure of ATP synthase under strain during catalysis by Hui Guo and John L. Rubinstein. Guo and Rubinstein, Structure of ATP synthase under strain during catalysis, 2022, Introduction and Figure 1: binding-change cycle
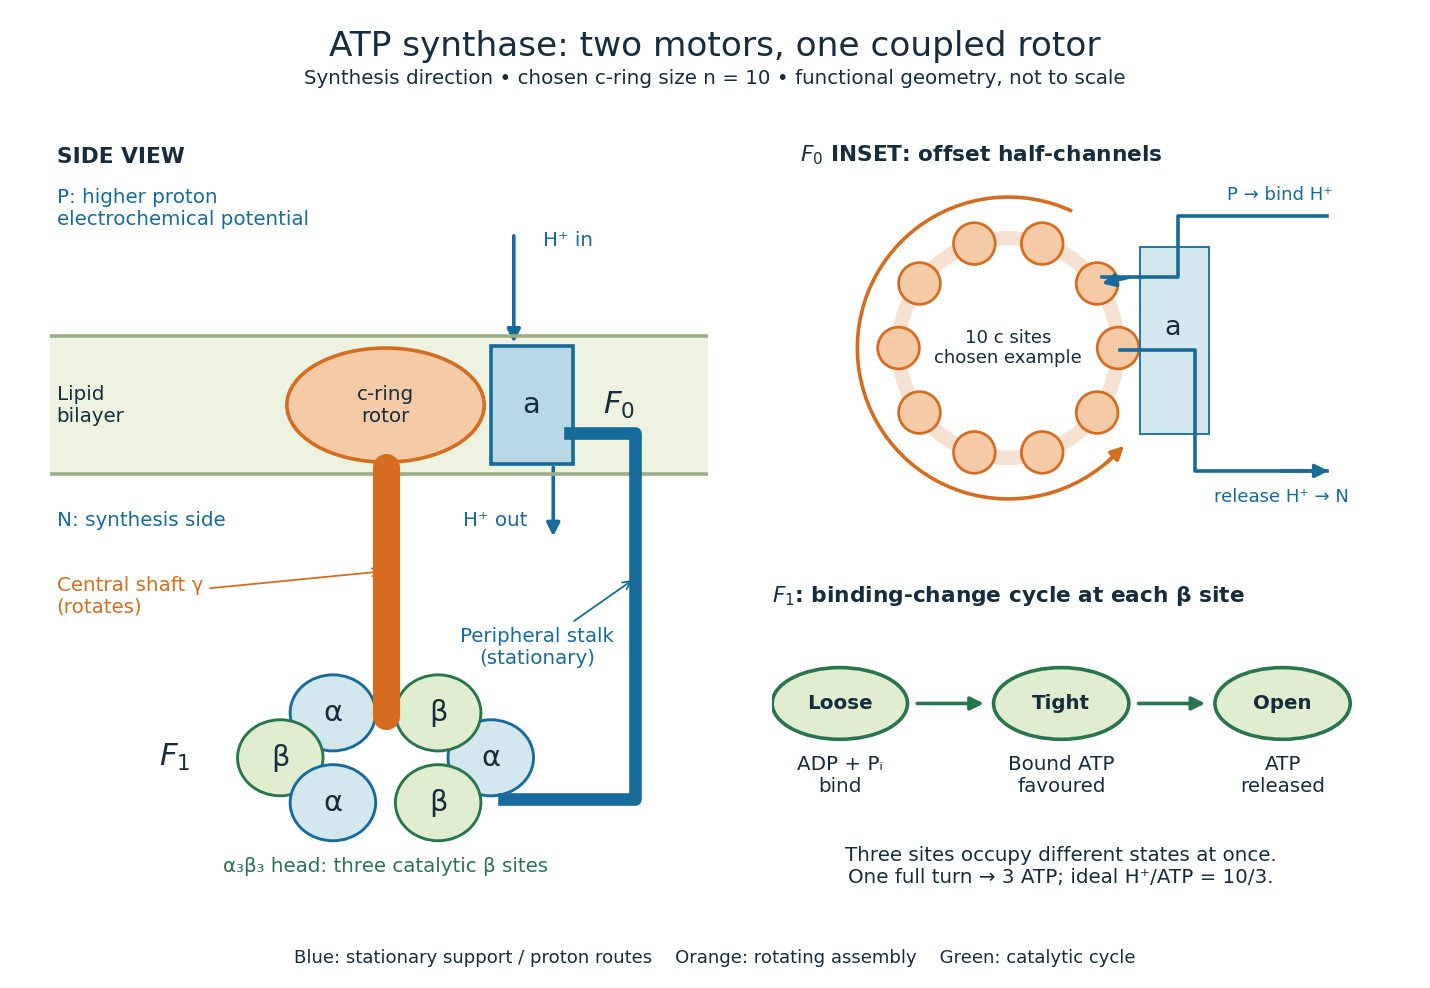
One complete, tightly coupled turn cycles each catalytic site once, producing three ATP molecules. If the ring has proton-binding subunits, the ideal motor budget is transferred protons per turn, or per ATP. Ring size varies between organisms; the worked example chooses , as in the studied bacterial systems, rather than assigning ten to every ATP synthase.[ref]
Rotary catalysis of FoF1-ATP synthase by Rikiya Watanabe. Watanabe, 2013, pp. 51–52: c-ring stoichiometry and H+/ATP ratio
For this example the ring's repeat angle is , whereas the three-site catalytic cycle repeats after . Their ratio is , not an integer. Counting complete turns avoids inventing a fixed integer proton count for every catalytic event. The schematic does not require both parts to advance simultaneously as rigid gears; elasticity allows temporary twisting while their cycles proceed.[ref]
Structure of ATP synthase under strain during catalysis by Hui Guo and John L. Rubinstein. Guo and Rubinstein, 2022, Introduction and Figure 1: symmetry mismatch and elastic coupling
Atomic Spectroscopy - A Compendium of Basic Ideas, Notation, Data, and Formulas by William C. Martin and Wolfgang Wiese 12. Zeeman Effect by Codex 0 2026-10-18
Codex 0 2026-10-18An isotope shift is a difference between corresponding atomic transition frequencies in different isotopes. One contribution comes from nuclear mass, through recoil and electron correlations; another comes from the changing nuclear charge distribution. For a specified transition, the leading finite-size contribution is often written , with an electronic factor . Extracting changes of nuclear charge radius therefore requires separating mass and finite-size contributions rather than identifying the entire shift with radius.
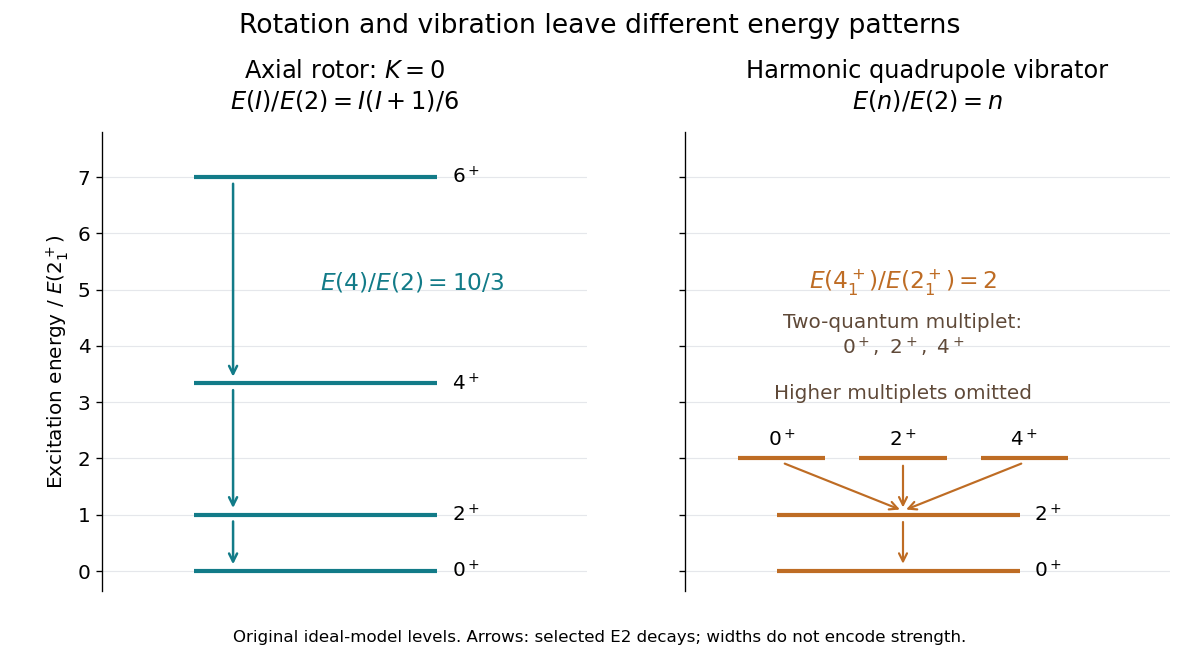
A sequence of nuclear energy levels interpreted as different total angular momenta built on approximately the same intrinsic structure. For an axially symmetric, positive-parity, ground state band of an even-even nucleus, the allowed sequence is . The simple constant-inertia rotor hasHere is an effective moment of inertia, and the reduced Planck constant. The even- restriction belongs to this particular intrinsic symmetry and band, rather than to all nuclear excitations. The angular momentum operator eigenvalue supplies , rather than the classical replacement .
Set . Since , the model predictsFor a chosen model scale , the excitation energies are . The corresponding successive gamma ray energies are approximately , neglecting nuclear recoil. Level energies and emitted line energies are different lists. These numbers illustrate the formula and are not a measured isotope spectrum.
The fitted is a response parameter, not automatically the moment of inertia of a classical rigid charge distribution. Nuclear pairing changes this response; Ben Roy Mottelson connected observed inertias with correlations beyond independent-particle motion.[ref]
Elementary Modes of Excitation in the Nucleus by Ben Roy Mottelson. continuation after p. 237, pairing correlations and Fig. 1 potential-energy surfaces
At larger angular momentum, changing intrinsic structure or nuclear pairing can invalidate a single constant . A useful diagnostic is to compare across several levels: constancy tests the simple formula, while a drift identifies the need for additional physics. A successful ratio alone neither specifies every microscopic motion nor measures a literal solid-body rotation.
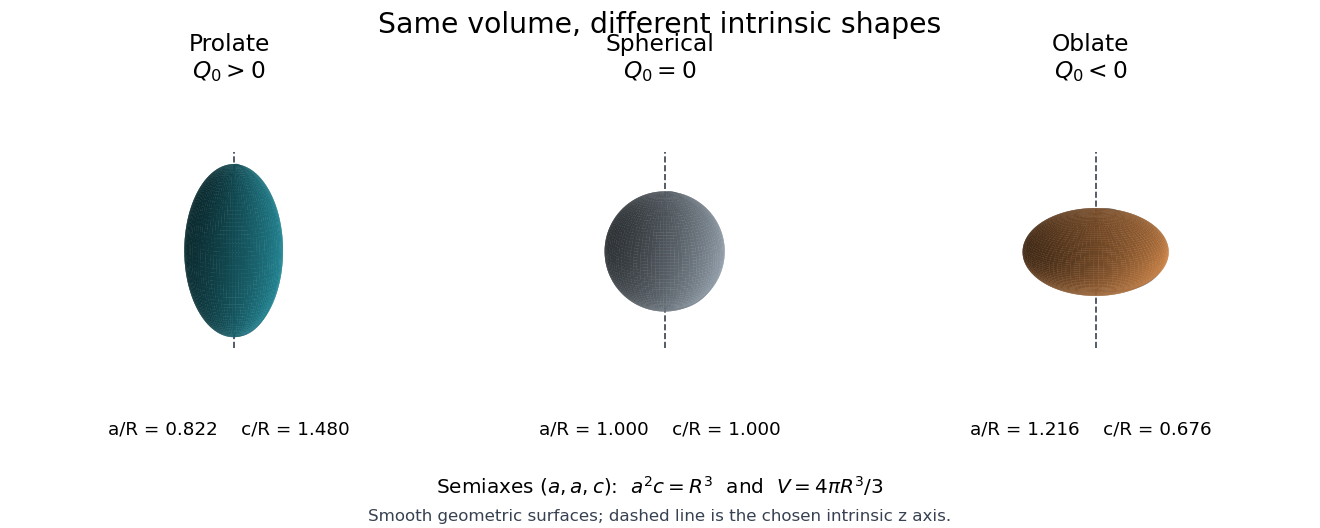
Departure of an intrinsic nuclear shape from spherical symmetry. Here intrinsic means referred to axes attached to a model nuclear charge distribution. A nuclear quantum state with definite spin need not have the same laboratory charge density as that intrinsic distribution. In particular, the ground state of a deformed even-even nucleus can have , a spherical laboratory expectation value, and a nonzero intrinsic nuclear quadrupole moment.
For an illustrative uniform charge density inside a spheroid, let the semiaxes be and keep its volume equal to that of a sphere of radius :Thus gives a prolate spheroid, a sphere, and an oblate spheroid. These are three-dimensional equal-volume shapes: equal areas of their drawn cross-sections would be a different constraint. Real nuclear charge distributions have diffuse surfaces and need not be uniform, axially symmetric or confined to one shape.
An atomic nucleus with even proton number and even neutron number . The simple nuclear pairing picture couples the constituent pairs to zero angular momentum. The collective examples below concern a ground state, where the superscript denotes positive parity, and its associated low-lying excitations; even alone would also allow odd and odd .
A description of an atomic nucleus in terms of coordinated motion of many nucleons, especially changes in shape and orientation. The nuclear shell model organizes individual nucleon states in a nuclear mean field; the collective nuclear model organizes low-lying energy levels by nuclear deformation, nuclear rotational bands and nuclear quadrupole vibrations. These are complementary organizations of the same nuclear many-body problem. A deformed nuclear mean field can support individual-particle states while its orientation supplies a slow collective coordinate.
In his 1975 lecture, Ben Roy Mottelson described coupling individual-particle motion to nuclear shape coordinates, and distinguished observed rotational spectra from vibrations about spherical equilibrium. This connects the two descriptions without treating the collective coordinates as extra constituent particles.[ref]
Elementary Modes of Excitation in the Nucleus by Ben Roy Mottelson. pp. 236–237, coupled Hamiltonian and interpretation of low-energy excitation spectra
James Rainwater's 1975 account identifies unexpectedly large electric quadrupole moments as a motivation for a deformable nuclear mean field. The challenge concerned their magnitude, even where spherical-shell trends had the correct sign.[ref]
Background for the Spheroidal Nuclear Model Proposal by James Rainwater. p. 264, Fig. 3 and discussion of the 1949 quadrupole compilation
A simple original potential energy example makes the coupling tangible. Let be a dimensionless signed shape coordinate for a chosen intrinsic configuration, its restoring stiffness, and a configuration-dependent coupling, both with units of energy. SupposeThe minimum is , with energy gain . For chosen values and , where is an arbitrary positive energy unit, and the gain is . This illustrates how a configuration can favor deformation when the core can respond. It is not a fitted nuclear surface or a claim that every configuration chooses the same shape; competing configurations and nuclear pairing can favor a spherical minimum.
The predictive attraction is economy: one collective scale relates several energy levels, while electric quadrupole transitions independently test their common structure. Agreement in both is much more restrictive than assigning a separate free parameter to every level. Nuclear magnetic moments test magnetic structure and angular momentum assignments; they are distinct observables from the electric quadrupole moments used to infer charge deformation.
Why should adding one neutron be easy for one atomic nucleus and much less favorable for its neighbor? In the nuclear shell model, nucleons occupy discrete energy levels in a nuclear mean field. Filling all available states below a sufficiently large gap produces a nuclear shell closure. This connects nuclear separation energies with the counting of quantum states, and connects the spin of an odd atomic nucleus with its last unpaired nucleon.
The starting point is an approximate Hamiltonian operatorwhere is a confining potential energy, specifies nuclear spin-orbit splitting, and contains interactions left out of the nuclear mean field. This is an effective organization of the nuclear many-body problem, rather than a derivation of the nuclear force. In a spherical approximation, addition of angular momentum combines the orbital angular momentum with spin to give ; for , only exists.
A level labelled has magnetic substates . The Pauli exclusion principle permits one neutron in each such state and, separately, one proton. Thus a level holds eight neutrons, or eight protons; it does not hold sixteen identical neutrons. Here counts radial levels of the same , starting with the lowest; it is not the hydrogenic principal quantum number. The letters mean .
Pinned article: Introduction to the OurBigBook Project
Welcome to the OurBigBook Project! Our goal is to create the perfect publishing platform for STEM subjects, and get university-level students to write the best free STEM tutorials ever.
Everyone is welcome to create an account and play with the site: ourbigbook.com/go/register. We belive that students themselves can write amazing tutorials, but teachers are welcome too. You can write about anything you want, it doesn't have to be STEM or even educational. Silly test content is very welcome and you won't be penalized in any way. Just keep it legal!
Intro to OurBigBook
. Source. We have two killer features:
- topics: topics group articles by different users with the same title, e.g. here is the topic for the "Fundamental Theorem of Calculus" ourbigbook.com/go/topic/fundamental-theorem-of-calculusArticles of different users are sorted by upvote within each article page. This feature is a bit like:
- a Wikipedia where each user can have their own version of each article
- a Q&A website like Stack Overflow, where multiple people can give their views on a given topic, and the best ones are sorted by upvote. Except you don't need to wait for someone to ask first, and any topic goes, no matter how narrow or broad
This feature makes it possible for readers to find better explanations of any topic created by other writers. And it allows writers to create an explanation in a place that readers might actually find it.
Figure 1. Screenshot of the "Derivative" topic page. View it live at: ourbigbook.com/go/topic/derivativeVideo 2. OurBigBook Web topics demo. Source. - local editing: you can store all your personal knowledge base content locally in a plaintext markup format that can be edited locally and published either:This way you can be sure that even if OurBigBook.com were to go down one day (which we have no plans to do as it is quite cheap to host!), your content will still be perfectly readable as a static site.
- to OurBigBook.com to get awesome multi-user features like topics and likes
- as HTML files to a static website, which you can host yourself for free on many external providers like GitHub Pages, and remain in full control

Figure 2. You can publish local OurBigBook lightweight markup files to either OurBigBook.com or as a static website.
Figure 3. Visual Studio Code extension installation.
Figure 5. . You can also edit articles on the Web editor without installing anything locally. Video 3. Edit locally and publish demo. Source. This shows editing OurBigBook Markup and publishing it using the Visual Studio Code extension. 
- Infinitely deep tables of contents:




All our software is open source and hosted at: github.com/ourbigbook/ourbigbook
Further documentation can be found at: docs.ourbigbook.com
Feel free to reach our to us for any help or suggestions: docs.ourbigbook.com/#contact