Epigenetic information affects plant genome evolution both by regulating the behavior of DNA sequences and by supplying heritable regulatory variation on which selection can act. It is therefore neither an alternative to genetic evolution nor merely a passive consequence of it. Changes in DNA methylation, chromatin and small-RNA targeting influence which sequences transpose, recombine, mutate or remain expressed, while the DNA sequence helps determine where those epigenetic states are established.
An epigenetic state is not simply a measurement of expression at one instant. For evolutionary purposes, one must ask whether a difference persists through cell division, survives reproduction and changes a phenotype relevant to reproductive success. An epiallele can differ in regulatory state without a change in the local nucleotide sequence, but many epigenetic differences are caused by genetic variation elsewhere. A newly inserted repeat, for example, may recruit silencing to a nearby gene. The insertion is a genetic difference, while the resulting methylation is part of its mechanism. Demonstrating an independent epigenetic contribution therefore requires more than finding different methylomes in genetically different varieties.
A major connection is control of transposable elements. Mobilization can increase copy number, interrupt coding sequences, change gene regulation and promote rearrangements between repeated sequences. plants silence many such elements through DNA methylation, H3K9me2 and RNA-directed DNA methylation. This protects genome integrity but also permits a genome to tolerate a reservoir of potentially mobile DNA. The physical accessibility of that DNA matters: DDM1 helps methyltransferases reach nucleosomal heterochromatin, showing how chromatin organization contributes to the containment of repetitive sequences.[ref]
The Arabidopsis nucleosome remodeler DDM1 allows DNA methyltransferases to access H1-containing heterochromatin by Assaf Zemach and others. experimental analysis of heterochromatic methylation and transposon regulation
Silencing is not permanently absolute. Failure or reprogramming of maintenance can expose an element to transcription, and a successful new insertion can create a lasting sequence change even if silencing is restored later. Reactivation in a somatic cell is not automatically evolutionarily transmitted: an insertion must reach a reproductive lineage to contribute directly to inherited genome change. In Arabidopsis thaliana pollen, transposon reactivation in the vegetative nucleus was distinguished from the protected sperm lineage; the associated small RNAs illustrated how one cell type can contribute information relevant to silencing in another.[ref]
Epigenetic reprogramming and small RNA silencing of transposable elements in pollen by R. Keith Slotkin and others. Summary and comparison of pollen vegetative nuclei with sperm
This is regulated reprogramming, not indiscriminate activation of the inherited genome.Transposon control also changes the material available for regulatory evolution. An insertion may carry a promoter, enhancer or transcription-factor binding site, while its epigenetic silencing can repress an adjacent gene or define a chromatin boundary. If selection favors part of the inserted sequence, its regulatory contribution can be retained while other element functions decay. Conversely, inappropriate spread of silencing can be harmful. The evolutionary outcome depends on insertion position, expression effects, mobility and host regulation; it is not true that all transposon activity is beneficial or that all methylation near genes is repressive. In particular, gene-body CG methylation and promoter-associated silencing should not be treated as interchangeable states.
Epigenetic information also influences sequence evolution through mutation and recombination. hydrolytic deamination of methylated cytosine can generate a thymine mismatch and, if unrepaired, a C-to-T substitution. A regulatory mark can thus change the probability of a subsequent genetic mutation; the resulting base substitution is no longer an epimutation. chromatin state also helps organize where meiotic breaks and crossovers occur. Repeat-rich heterochromatin often exchanges less readily than gene-rich chromosome arms, altering the degree to which selection acts on linked variants. These effects are contextual rather than a rule that every methylated cytosine or every marked region has the same evolutionary fate.
There is also a genuinely heritable state component. Mutation-accumulation lines of Arabidopsis thaliana showed spontaneous methylation differences across generations, with individual sites more labile than many larger methylated regions and with recurrent changes at some sites.[ref]
Spontaneous epigenetic variation in the Arabidopsis thaliana methylome by Claude Becker and others. comparison of lines descended from a common ancestor; regional stability and recurrent epimutations
Thus an epigenetic variant's evolutionary importance depends jointly on its phenotypic effect, transmission probability and reversion rate. A rapidly reversible state may support plasticity but fail to behave like a stable DNA allele over many generations.Experiments with epigenetic recombinant inbred lines provide evidence that some methylation differences can contribute to quantitative phenotypes. Mapping in a comparatively uniform genetic background identified epigenetic loci associated with flowering time and root length.[ref]
Mapping the epigenetic basis of complex traits by Sandra Cortijo and others. epigenetic quantitative-trait mapping and selection in epiRILs
This establishes a possible substrate for selection, not a claim that most natural adaptation is sequence-independent. Residual sequence variation, new transposon insertions, genetic control of methylation and environment-dependent effects must still be distinguished in natural populations.Hybridization and allopolyploidy create further interactions. Divergent regulatory systems and multiple parental copies must operate together, and changes in chromatin can alter dosage or expression before any gene is lost. In nucleolar dominance, one parental set of ribosomal RNA genes is epigenetically silenced. The involvement of HDA6, DNA methylation and histone-state changes shows that unequal parental expression can arise without deleting the silent set.[ref]
Erasure of histone acetylation by Arabidopsis HDA6 mediates large-scale gene silencing in nucleolar dominance by Keith Earley and others. Abstract and perturbation of parental rRNA-gene silencing
Such expression differences can influence which duplicate functions remain useful, although silencing alone does not prove the later direction of gene loss or subgenome evolution.Epigenetic information therefore shapes genome evolution as a regulator of genome activity, a modifier of genetic change and sometimes an inherited source of phenotypic variation. Its effects must be analyzed together with sequence, reproduction and selection, without assuming that environmentally induced changes are necessarily adaptive or permanently inherited.
Epigenetic modification could improve a crop by selecting useful stable regulatory variants, deliberately altering a validated locus, preserving favorable states during propagation, or exploiting temporary physiological memory when permanent inheritance is unnecessary. The appropriate strategy depends on the trait, the crop's mode of propagation and the stability of the state. A useful methylation marker is not automatically a causal target, and a demonstration in Arabidopsis thaliana is not yet an improved field variety.
A sensible starting point is natural variation. A breeder can relate a phenotype to differentially methylated regions, while measuring genotype, expression and relevant environmental history. epigenome-wide association studies can prioritize candidate loci, but local sequence differences, trans-acting regulators and differences in tissue composition can all produce methylation associations. Common-environment comparisons, reciprocal crosses where appropriate and evidence that changing the state changes the trait help establish causation. The desired product is a regulatory state that remains useful in the target genetic background, not simply the largest statistical methylation difference.
A concrete nutritional example is VTE3(1) in tomato. Differential methylation associated with a promoter retrotransposon affects expression of a vitamin E biosynthetic gene and fruit tocopherol accumulation. The reported epialleles connect a regulatory state with an agronomic quality trait, rather than merely correlating bulk methylation with vigorous growth.[ref]
Natural occurring epialleles determine vitamin E accumulation in tomato fruits by Leandro Quadrana and others. Abstract; promoter methylation, expression and fruit tocopherol analyses
Selecting a favorable state could therefore complement conventional selection, provided its stability, the underlying promoter sequence and any correlated quality effects are characterized. The existence of this example does not imply that removing methylation generally raises crop quality.A second route is to create and select broader epigenetic variation. Transient disruption of methylation maintenance can generate epigenetic recombinant inbred lines after the initiating genetic defect is removed. Such populations have produced selectable variation in quantitative traits in Arabidopsis thaliana.[ref]
Mapping the epigenetic basis of complex traits by Sandra Cortijo and others. epiRIL trait mapping and response to selection
They can reveal regulatory states not readily encountered in an existing breeding pool. However, broad hypomethylation can also activate transposons or destabilize development. Genome sequencing is needed to distinguish genuine state effects from new insertions or other mutations, and restoring a maintenance gene does not guarantee that every induced epiallele will persist.somaclonal variation during tissue culture is another source of altered states, but a good crop strategy can involve preventing harmful epigenetic change rather than generating more. In African oil palm, loss of methylation at the Karma epiallele in an intronic retrotransposon is associated with abnormal splicing, mantled flowers and reduced yield. Methylation near the relevant splice region provided a predictor of the damaging variant.[ref]
Loss of Karma transposon methylation underlies the mantled somaclonal variant of oil palm by Meilina Ong-Abdullah and others. Abstract and relation between methylation, transcript processing and fruit phenotype
Screening propagated material for the favorable state can protect the value of elite clones; it is not evidence that arbitrary stress-induced methylation will improve yield.More directed approaches use epigenome editing. A sequence-targeting protein such as dCas9 can recruit an activity that changes DNA methylation or a chromatin regulator, rather than cutting the target sequence. One can in principle tune a validated promoter's expression while retaining its coding sequence. Targeted demethylation of the FWA locus in Arabidopsis thaliana demonstrated that a changed methylation state can alter expression and flowering behavior, with inheritance of the state at that particular locus.[ref]
Targeted DNA demethylation of the Arabidopsis genome using the human TET1 catalytic domain by Javier Gallego-Bartolomé and others. FWA-targeted demethylation, expression, flowering and inheritance tests
This is a proof of a mechanism, not a recommendation that delayed flowering is universally favorable or that every edited locus will retain its state after the targeting factor disappears.The causal chain should guide target choice: a defined regulatory state changes expression in the relevant tissue, which changes a biochemical or developmental process, which improves the intended crop trait. Possible objectives include modifying flowering schedules, improving nutritional composition or reducing an unfavorable expression state during clonal propagation. Persistent effects require a mechanism for maintaining the new state. If local DNA repeats or small-RNA pathways continually restore the original state, a transient edit may be erased. Conversely, a state that is too persistent may impair later developmental transitions. Specificity also matters because broad changes to a chromatin enzyme affect many loci simultaneously.
Not every useful application requires an inherited epiallele. Seed priming or a prior acclimating exposure can change later stress responses within the same crop generation. If the treatment reproducibly improves establishment under the intended conditions, it can be agronomically useful even when offspring return to the original state. Nevertheless, stress priming may be mediated by stored metabolites, hormones or proteins rather than inherited chromatin. Benefits can disappear in another environment or be offset by reduced growth, altered maturation or shorter seed storage life. Such treatments should be evaluated as defined management interventions, rather than being advertised as proven transgenerational breeding.
Any deployment needs tests matched to how the crop is propagated. A seed-propagated line must transmit the favorable effect through reproduction; a clone must retain it through the relevant number of propagation cycles. Multi-environment trials should measure the intended endpoint and relevant costs, including fertility, developmental normality and yield stability. Comparing treated and untreated material of the same genotype, checking independent derivations and monitoring sequence as well as epigenetic state reduce the risk of attributing an unrelated change to the proposed mechanism. Molecular differences alone do not establish an economic benefit.
The strongest strategy is therefore to treat epigenetic state as an additional, testable breeding or management variable. Natural epialleles, directed editing and propagation control offer different opportunities, but none removes the need to establish causality, persistence and benefit in the actual crop and production environment.
plants establish epigenetic states through sequence- and context-dependent recruitment, maintain selected states through replication and regulatory feedback, and erase others when development requires a reset. These processes protect repetitive DNA, stabilize cell identity and coordinate developmental or environmental responses. An epigenetic state is therefore regulated information, not simply a collection of chemical marks that always switch genes off.
plant DNA methylation occurs in CG, CHG and CHH contexts, where H denotes A, C or T. The contexts have overlapping but distinct control mechanisms. At a methylated CG dyad, DNA replication initially produces hemimethylated daughter DNA; MET1 helps restore methylation on the new strand. This provides a direct route for maintaining an existing pattern. By contrast, asymmetric CHH methylation cannot be retained merely by copying an equivalent methylated cytosine across a symmetric dyad: continued targeting by small-RNA or chromatin pathways is required. CHG methylation is strongly coupled to histone recognition and reinforcing chromatin feedback rather than being explained by CG maintenance alone.
For establishment at many repeats, canonical RNA-directed DNA methylation provides sequence specificity. Pol IV produces precursors that, with RDR2, generate double-stranded RNA; DCL3 processes these into 24-nucleotide small interfering RNAs. An Argonaute such as AGO4 uses guide information in association with nascent scaffold transcripts made by Pol V, helping recruit DRM2 to the matching locus. DRM2 can establish methylation in multiple cytosine contexts. Thus transcription can paradoxically be required to establish transcriptional silencing: the scaffold supplies a locus-specific interaction surface rather than representing productive expression of the silenced gene.[ref]
Pol IVb and Pol V noncoding-transcription study by Andrzej T. Wierzbicki and others. Pol V scaffold transcription and its requirement alongside siRNA production
Maintenance is also reinforced by interactions between DNA and histone states. CMT3 recognizes H3K9me2-associated chromatin and contributes to CHG methylation. Histone methyltransferases including SUVH4, SUVH5 and SUVH6 couple methylated DNA to H3K9 methylation, forming a reinforcing relationship. CMT2 contributes strongly to CHH methylation in heterochromatic regions, while RdDM is particularly important in other targeted contexts. Mutant methylomes show both specialization and redundancy, as well as dependencies linking non-CG methylation, small RNAs and H3K9 states.[ref]
Non-CG methylation patterns shape the epigenetic landscape in Arabidopsis by Hume Stroud and others. methyltransferase mutants, CMT2 activity and dependencies between epigenetic pathways
These are interacting pathways, not three enzymes independently copying three unrelated codes.Accessibility is an essential part of the mechanism. Dense nucleosomes and linker histones can restrict a methyltransferase even when an appropriate DNA sequence is present. DDM1 remodels H1-containing heterochromatin to allow access, complementing RNA-directed targeting in different chromatin environments.[ref]
The Arabidopsis nucleosome remodeler DDM1 allows DNA methyltransferases to access H1-containing heterochromatin by Assaf Zemach and others. heterochromatin accessibility and complementary methylation pathways
This explains why maintenance can depend on both an enzyme that writes a modification and machinery that permits the enzyme to reach its substrate.Histone-based developmental memory is a distinct layer. Polycomb repressive complex 2 deposits H3K27me3 at selected developmental loci. Sequence-specific regulators, transcriptional context and environmental signals determine where recruitment occurs; recycling of parental histones and restoration of modifications help preserve selected states after replication. Yet the presence of a histone mark does not prove that the mark autonomously copies itself or is sufficient for inheritance. Recruitment, feedback, nucleosome turnover and the transcriptional state all need to be considered. H3K27-based silencing of developmental genes should also be distinguished from H3K9-associated transposon heterochromatin.
vernalization illustrates how a state is established for a purpose and maintained for a limited interval. In Arabidopsis thaliana, prolonged cold promotes stable repression of the floral repressor FLC, allowing later flowering in appropriate conditions. Natural accessions differ in the cold exposure needed for stable silencing, correlated with accumulation of H3K27me3.[ref]
Variation in the epigenetic silencing of FLC contributes to natural variation in Arabidopsis vernalization response by Chikako Shindo and others. variation in stable FLC silencing and H3K27me3 after different cold exposures
Maintaining the state after warming allows the plant to retain information about winter rather than respond only to the instantaneous temperature.Erasure is equally important. Active DNA demethylation can involve DNA glycosylase/lyase activity followed by repair that replaces methylated bases. The identification of ROS1 connected promoter demethylation to protection against inappropriate gene silencing.[ref]
ROS1 gene-silencing study by Zhizhong Gong and others. ROS1 mutant phenotype and methylated-DNA glycosylase activity
Reproductive reprogramming is cell-type specific: DEMETER has a maternal role in imprinting and seed viability, rather than representing indiscriminate erasure in every cell.[ref]An environmentally acquired state may also need resetting between generations. The vernalized FLC state is normally reset during reproduction and seed development, so the offspring can require its own winter. Perturbing the histone demethylase ELF6 impaired resetting and allowed inheritance of a partially vernalized state.[ref]
Epigenetic reprogramming that prevents transgenerational inheritance of the vernalized state by Pedro Crevillén and others. FLC resetting and ELF6-dependent H3K27 demethylation
This contrasts with loci whose methylation states remain stable through reproduction. plants cannot be described either as preserving every acquired mark or as globally erasing all epigenetic information.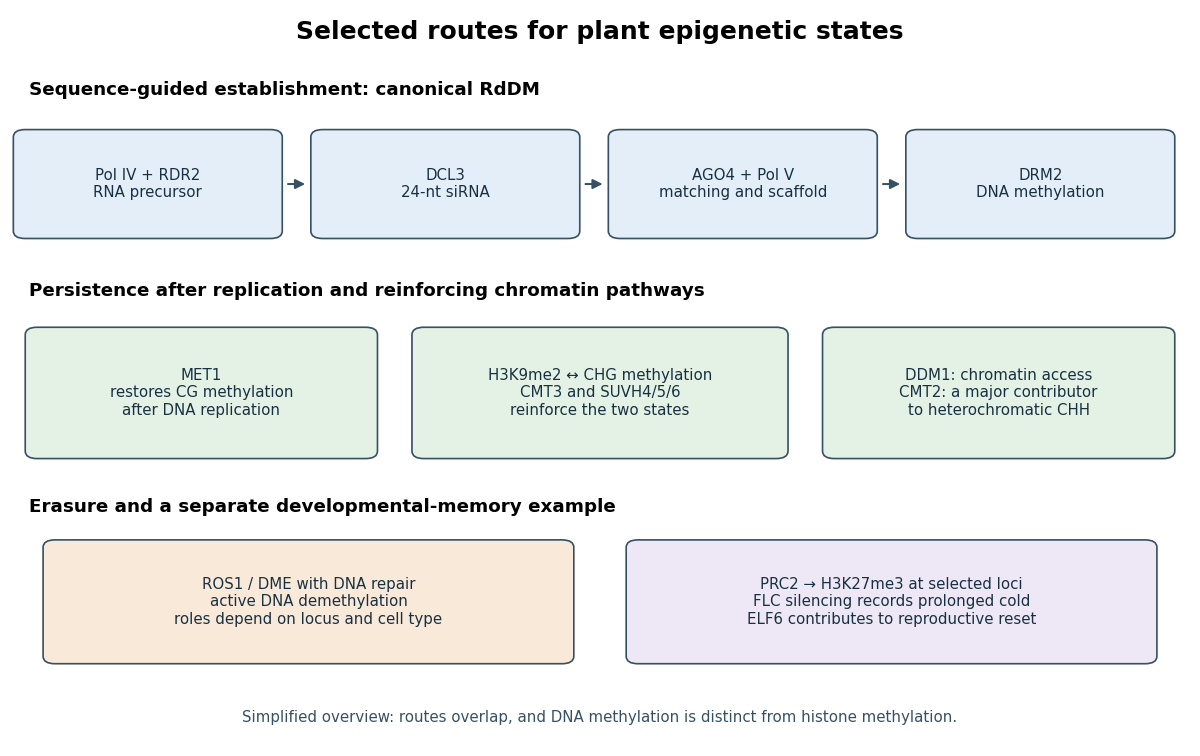
Original overview of DNA methylation establishment, reinforcing maintenance, active demethylation and a distinct Polycomb developmental-memory pathway
. Details. 
Why retain these systems? Silencing mobile and repetitive DNA limits genome damage, chromatin states help cells maintain appropriate expression despite a shared genome, and developmental memory coordinates events separated in time. Selective reprogramming supports gametes and seeds, while boundaries and active demethylation prevent necessary silencing from spreading into genes that must function. Methylation within an expressed gene is not equivalent to repression at a promoter, and a transient transcriptional response is not automatically an inherited state. plant epigenetic control is therefore a balance of targeting, faithful persistence and timely erasure, with different mechanisms serving different biological intervals and genomic contexts.
A crop's future performance depends on its past because development, stored resources and environmental experience change what the plant or its offspring can do next. Some effects are transient physiological carry-over, some involve stable somatic chromatin states, and a smaller set may persist through reproduction. Life-history strategy—especially annual versus perennial growth—also determines whether a response that helps now benefits later reproduction or harvest.
Development creates sequential competence. Germination, juvenile growth, reproductive transition and seed filling are not interchangeable stages: exposure to the same stress at each stage can have different consequences. Early damage can reduce leaf area or root capacity and therefore later yield even after the original stress disappears. Carbon reserves, nutrient stores, root architecture and meristem condition can all carry information about the past without requiring an epigenetic mechanism. A study claiming memory must distinguish those persistent physical consequences from a changed response to a genuinely new challenge.
A clear beneficial memory is vernalization. In plants requiring winter cold, the past temperature sequence affects later flowering under otherwise similar warm conditions. In Arabidopsis thaliana, cold-induced repression of FLC can remain after warming, while different accessions require different durations of cold for reliable silencing.[ref]
Variation in the epigenetic silencing of FLC contributes to natural variation in Arabidopsis vernalization response by Chikako Shindo and others. accession-dependent cold requirements and stable repression after warming
The ecological value is seasonal coordination: responding to a brief warm interval without sufficient winter experience could expose reproduction to damaging conditions. In crops, sowing date, cultivar requirement and local winter history consequently interact to determine flowering and the time available for grain filling.The exact mechanism should not be generalized across all crops. FLC-based regulation is a well-characterized Arabidopsis thaliana example; cereal vernalization networks use different core regulators. The common functional issue is how a record of past cold is integrated with current temperature, day length and developmental competence. Nor is vernalization necessarily a useful inherited gift to offspring. FLC normally resets during reproduction, so a new generation evaluates its own season; defective ELF6-dependent resetting demonstrated that failure to erase the state can permit partial inheritance.[ref]
Epigenetic reprogramming that prevents transgenerational inheritance of the vernalized state by Pedro Crevillén and others. resetting of FLC and the elf6 resetting mutant
A state can be valuable within a lifetime precisely because it is not transmitted indefinitely.annual plants and perennial plants face different future demands. An annual grain crop must balance vegetative growth against completing reproduction in the current season. A perennial must also preserve meristems and resources for survival and later reproductive episodes. In the perennial Arabis alpina, PEP1, an FLC orthologue, is reactivated after cold and helps restrict flowering duration and preserve vegetative branches.[ref]
PEP1 regulates perennial flowering in Arabis alpina by Renhou Wang and others. PEP1 seasonal expression and effects on flowering duration and vegetative growth
This model-system comparison shows why an epigenetic switch optimized for one reproductive episode may be unsuitable for repeated flowering. For perennial crops, current harvest can also affect next-season reserves, so one-season yield alone can misrepresent performance.Past stress can change a later response through stress priming. After an initial exposure and recovery interval, a plant may retain defense-related proteins, metabolites or regulatory changes that make a subsequent response faster or stronger. In Arabidopsis thaliana heat-memory experiments, HSFA2 was required for sustained transcriptional memory and associated accumulation of H3K4 methylation at selected loci after the initial response.[ref]
A hit-and-run heat shock factor governs sustained histone methylation and transcriptional stress memory by Jörn Lämke and others. HSFA2 dependence, persistent H3K4 methylation and recurrent heat responses
This provides a mechanistic example of somatic stress memory, not proof that all crop stresses produce a beneficial heritable epiallele.The benefits depend on the future environment. Maintaining readiness costs resources and may compromise growth if the predicted stress never returns. Priming against one challenge may not protect against another; severe first exposure can cause lasting injury rather than useful preparation. The interval between exposures and the organ being measured also matter. A well-designed comparison therefore includes an initial-exposure-only group, a challenge-only group, a primed-and-challenged group and an appropriate untreated control, with performance measured after accounting for developmental differences. Improved survival alone is not equivalent to improved harvest yield.
Parental history adds another layer. The environment of a seed-producing plant can alter seed size, nutrient provisioning, hormone balance, seed coat properties and dormancy. In Arabidopsis thaliana, maternal temperature history affected progeny dormancy through regulation involving FLOWERING LOCUS T in fruit tissues.[ref]
Maternal temperature history activates Flowering Locus T in fruits to control progeny dormancy according to time of year by Min Chen and others. Abstract; maternal temperature, fruit FT activity and progeny dormancy
Such a maternal effect is biologically important even if no chromatin mark passes through the embryo. In seed production, apparently identical cultivars can consequently establish differently because of conditions during seed maturation and storage.This makes evidence for transgenerational epigenetic inheritance demanding. An effect in offspring can reflect direct exposure of developing seeds, maternal provisioning, transmitted microbes or an unrecognized DNA variant. Effects must persist beyond directly exposed generations under controlled conditions, with genetic and parental alternatives addressed, before being described as inherited epigenetic memory. Reciprocal crosses and comparisons of independently propagated families can help distinguish alternatives, but a methylation difference alone does not identify the causal route.
Clonal crop propagation changes the relevant horizon. A somatic state may pass directly through cuttings, grafts or tissue culture without meiosis, making within-lineage persistence economically important. Tissue culture can also introduce harmful states: the methylation-associated Karma epiallele in African oil palm connects propagation history with later fruit abnormalities and yield loss.[ref]
Loss of Karma transposon methylation underlies the mantled somaclonal variant of oil palm by Meilina Ong-Abdullah and others. somaclonal origin and methylation-associated mantled phenotype
Conversely, a seed treatment that improves rapid emergence may reduce storage longevity, so seed vigor should be evaluated in the actual production and storage system.Life history thus affects future crop performance through developmental timing, persistent physiology, somatic memory and parental effects, interpreted within the crop's reproductive strategy. The agronomic task is to identify which past events matter, how long their effects last, and whether they improve the particular future outcome being optimized.
Crossover limitations can be addressed by changing recombination number, changing its genomic distribution, or overcoming barriers between the chromosomes being crossed. Genetic and epigenetic approaches act on different parts of this problem and can complement each other. The breeding objective is a desired, fertile recombinant, not the largest genome-wide crossover count.
chromosomal crossovers exchange information between homologues during meiosis and allow favorable alleles to be combined while reducing linkage drag from an introgressed segment. However, a chromosome's physical length does not determine where useful crossovers occur. Large repeat-rich and pericentromeric regions may recombine poorly, while many events occur in restricted gene-rich regions. Structural differences, sequence divergence and, in polyploids, partner-choice mechanisms impose further barriers. Increasing events in an already recombination-rich arm may do little for a desired allele locked in a cold region.
Mechanistically, initiating Spo11-dependent DNA breaks is only the first step. Many breaks are repaired without reciprocal crossover, and the designation and maturation of crossover intermediates are tightly controlled. class I crossovers are subject to crossover interference, whereas class II crossovers provide a comparatively noninterfering route. crossover assurance helps maintain the connections needed for balanced homolog segregation. A modification that generates more breaks but leaves repair or chromosome pairing defective can therefore reduce fertility rather than improve breeding.
One genetic approach increases pro-crossover activity. Natural variation and dosage of the E3 ligase HEI10 affect crossover recombination in Arabidopsis thaliana, providing an example of a trans-acting modifier rather than a local sequence hotspot.[ref]
Natural variation and dosage of the HEI10 meiotic E3 ligase control Arabidopsis crossover recombination by Piotr A. Ziolkowski and others. HEI10 dosage and crossover measurements
This can increase the pool of recombinant products, but interference, local chromatin and chromosome structure still constrain where events mature. A beneficial effect must be tested in the target hybrid background rather than assumed from the model species.Another route weakens anti-crossover activities. RECQ4, FANCM and FIGL1 regulate the processing of meiotic intermediates, with different phenotypic effects across plant contexts. Disruption of RECQ4 orthologues increased crossovers by about threefold in rice, pea and tomato hybrids in the reported experiments.[ref]
Unleashing meiotic crossovers in crops by Delphine Mieulet and others. comparative RECQ4 analysis in rice, pea and tomato
This is direct crop evidence for relaxing one limit. It does not establish that every anti-crossover mutation works equally well, that combinations remain fertile, or that recombination is released uniformly across the genome. Extra events can also disrupt favorable linked combinations, so later breeding selection remains essential.Epigenetic approaches address the chromatin landscape. DNA methylation, H3K9me2 and nucleosome organization influence access to meiotic break formation and the subsequent probability of crossover. In Arabidopsis thaliana, disruption of H3K9 and non-CG methylation pathways, including CMT3 and SUVH4, SUVH5 and SUVH6, increased recombination near centromeres. The study combined break-related measurements with cytological crossover markers and genotyped recombinants, rather than inferring crossover gain from open chromatin alone.[ref]
The distinction between redistribution and total increase is crucial. A methylation perturbation can move crossovers from one region to another without increasing their total number, and loss of CG methylation need not have the same effect as disrupting non-CG/H3K9 pathways. More initiating breaks need not become crossovers. Moreover, repeat-rich regions and the functional centromere are not interchangeable: an increase in pericentromeric events does not mean that crossing over can safely be allowed everywhere. Suppression close to centromeres also helps preserve chromosome segregation.
For breeding, locus- or stage-specific chromatin manipulation is an attractive aim because it might alter accessibility near a desired target without permanently destabilizing the rest of the genome. Nevertheless, this remains an aim to validate rather than a universal solution. Broad demethylation can derepress transposons, alter expression and affect gamete quality. A local epigenetic change may be restored by maintenance pathways before meiosis, and modifying a region's accessibility does not remove an inversion or create homology that is absent. Combining a crossover-promoting genetic background with a justified local chromatin change is mechanistically plausible, but its value must be established by mapping actual transmitted crossovers.
Partner choice is a separate genetic limitation. In bread wheat, the Ph1 locus contributes to meiotic stability and limits exchange between related homoeologous chromosomes. Relaxing this control can facilitate homoeologous recombination useful for introgressing material from relatives, but it also changes the risk of inappropriate pairing or unbalanced products.[ref]
Dual effect of the wheat Ph1 locus on chromosome synapsis and crossover by Azahara C. Martín and others. homologue/homoeologue discrimination, synapsis and crossover outcomes
Structural compatibility and fertility therefore need assessment alongside the desired donor segment. In inversion heterozygotes, recovery of balanced recombinants can remain limited even if meiotic breaks become more frequent.The practical value can be expressed in terms of the target gamete's probability. If two desired alleles are in repulsion, , and the interval has recombination fraction , an idealized model gives the desired recombinant probability . Among independent sampled gametes,For , and at least 2995 gametes are needed for a 95% chance under this model. Increasing useful recombination can therefore reduce screening costs greatly, but crossover counts elsewhere do not change this calculation. Actual progeny designs must also account for mating scheme, viability and transmission distortion.
A successful strategy therefore measures where extra crossovers occur, whether they produce the intended haplotype and whether that haplotype is transmitted by fertile plants. Genetic pathway changes, epigenetic redistribution and partner-choice control solve related but distinct constraints; none removes the need for genotype-specific validation and selection.
Resistance-gene evolution reflects recurrent pathogen selection acting within ecological and physiological constraints, while duplication, sequence exchange and gene loss generate changing receptor repertoires. The result is not one universal genome organization: some receptors occur in variable clusters or linked functional pairs, others are conserved or dispersed, and some lineages lose parts of an immune pathway.
The relevant genes should first be distinguished. Pattern recognition receptors at the cell surface detect conserved microbial or damage-associated features, whereas many intracellular nucleotide-binding leucine-rich repeat receptors detect pathogen-derived molecules or disturbances of host targets. NLRs are a major class of resistance genes, but they are not all resistance genes: transport, metabolism, cell-wall properties and quantitative regulatory differences can also alter disease. Thus counts of NLRs describe one important part of the defense system rather than a complete measure of immunity.
Pathogens impose changing selection because recognition can reduce infection while successful pathogen variants evade or suppress the recognized response. A new recognition specificity can rise when it is useful; its advantage can decline when the corresponding pathogen population changes. Spatial and temporal variation in pathogen communities, and negative frequency-dependent selection under appropriate host–pathogen dynamics, can help maintain alternative resistance alleles through balancing selection. These processes need not produce the same signal as repeated directional selection. Conserved signaling functions may remain under purifying constraint while recognition-associated regions diversify more rapidly.
Resistance also has costs. Constitutive or inappropriate immune activity can divert resources, damage tissues or reduce reproduction in the absence of the relevant disease. This growth-defense trade-off makes loss or reduced expression of an unused receptor potentially advantageous, and means that greater gene number is not automatically better. Hybrid necrosis supplies a particularly clear constraint: combining alleles from otherwise viable parents can inappropriately activate immunity. A characterized Arabidopsis thaliana incompatibility involved an NLR-associated immune response, illustrating how combinations beneficial or harmless in their native backgrounds can become deleterious in hybrids.[ref]
The genomic raw material is generated by gene duplication, including tandem duplication, followed by divergence, deletion or pseudogenization: birth-and-death evolution. Unequal exchange and gene conversion can create copy-number differences and mosaic receptor sequences. A cluster therefore provides opportunities for new recognition combinations, while linked copies can also recombine into nonfunctional or incompatible products. Gene content may differ enough between accessions that a single reference genome omits relevant resistance loci altogether. Selection acts on the resulting haplotypes as well as on individual point substitutions.
Long-read, multi-accession analyses make that organization visible. The species-wide Arabidopsis thaliana NLR inventory found substantial presence-absence variation and architectural diversity, establishing the importance of a pan-NLRome rather than one reference receptor list.[ref]
A species-wide inventory of NLR genes and alleles in Arabidopsis thaliana by Anna-Lena Van de Weyer and others. species-wide inventory, presence-absence variation and integrated-domain diversity
Such variation is consistent with duplication, turnover and selection, but differences in assembly quality or annotation can also alter apparent counts. Comparative conclusions therefore require sufficiently complete genomes and consistent identification of intact genes and fragments.Physical linkage can preserve a functional combination as well as generate diversity. In a paired NLR system, recognition and downstream activation can be partitioned between partners. Selection can favor inheritance and coordinated expression of a compatible pair; indiscriminate recombination is then potentially harmful. The Arabidopsis thaliana RRS1-RPS4 receptor pair illustrates an integrated decoy mechanism, where a receptor-associated WRKY domain links perturbation of a target-like domain to immunity.[ref]
A receptor pair with an integrated decoy converts pathogen disabling of transcription factors to immunity by Clémentine Le Roux and others. paired receptor function and the integrated WRKY-domain mechanism
This is an explanation for one type of organization, not a rule that every cluster is a functional pair or every integrated domain has the same role.plant lifestyle changes the selection regime. A long-lived perennial can experience many pathogen seasons, making maintenance of effective defense across time important; an annual may sometimes escape a disease through seasonal timing. These are conditional expectations, not deterministic predictions of NLR counts. selfing changes heterozygosity and the persistence of linked combinations, while outcrossing exposes alleles to new partners and can favor different balances between recombination and linkage. Clonal propagation preserves whole immune haplotypes but can also produce large areas of similar susceptible hosts. crop domestication, breeding bottlenecks and uniform deployment consequently alter the evolutionary setting relative to a diverse wild population.
Ecological adaptation can also change which components are retained. Aquatic or otherwise specialized habitats differ in microbial exposure and in the physiological demands placed on a plant; symbiotic associations add selection against indiscriminate defense activation. Comparative work identified independent losses of NLRs together with EDS1/PAD4-associated signaling components in several plant lineages, with links to other immune and drought-response functions.[ref]
EDS1 and PAD4 pathway-loss study by Erin L. Baggs and others. comparative genome analyses and coordinated pathway loss
This supports pathway coevolution and rewiring. It does not prove that an aquatic lifestyle alone caused each loss, or that those species have no remaining defenses; phylogeny and additional ecological changes must be considered.Genomic organization therefore records both opportunity and constraint. Clusters can accelerate receptor-family turnover, linked pairs can preserve coadapted functions, and distributed signaling partners can limit which new sensors are useful. Changes in receptor expression, copy number and regulation may matter as much as coding-sequence diversity. Interactions with abiotic stress and beneficial microbes make pathogen pressure only part of the fitness landscape. Testing an evolutionary explanation requires connecting a genomic pattern to phenotype and ecology, rather than inferring selective benefit from a large cluster alone.
The resulting resistance genome is a dynamic, population-level repertoire shaped by pathogen variation, the costs of immune activation and the plant's ecological and reproductive context. This explains simultaneous rapid diversification, retention of compatible gene combinations and repeated gene loss, and why a resistance allele that is useful in one crop background or environment may not remain useful everywhere.
We understand several calcium sensors and downstream responses, but do not yet possess a general, predictive account of how a particular calcium signature selects a particular plant response. The unresolved problem is the causal transformation from a multidimensional signal to an outcome in its cellular context. It is too strong to say that nothing is known about calcium signal decoding.
A calcium signature includes the amplitude, duration, frequency and spatial distribution of increases in free calcium ion concentration. The nucleus, cytosol and regions close to ion channels can experience different signals. A stimulus may therefore change several candidate information-bearing variables simultaneously. Two treatments producing different oscillation frequencies might also differ in pulse height, total calcium exposure or the number of responding cells. A correlation between frequency and gene expression does not establish that frequency is the variable actually decoded. Nor need each stimulus have one unique calcium signature: different stimuli can recruit overlapping machinery, while the same stimulus can produce different responses in different tissues.
There are plausible molecular decoders. Calmodulin changes its interactions with targets after calcium binding. A calcium-dependent protein kinase combines a calcium sensor with a catalytic domain, directly connecting calcium binding to target phosphorylation. Calcineurin B-like proteins recruit CBL-interacting protein kinases, providing combinations of sensor, kinase and subcellular localization. In symbiotic signaling, nuclear oscillations feed into CCaMK and downstream developmental regulation. These mechanisms explain how calcium can influence an output; identifying one does not automatically explain discrimination among different waveforms.
Calcium sensor kinetics provide one possible mechanism. For a deliberately simplified sensor with active fraction , free calcium concentration and positive rate constants, considerWhen calcium returns to a negligible value between pulses, decays approximately as . Pulses separated by much less than can therefore accumulate sensor activation; widely separated pulses allow recovery. This is an illustrative kinetic model, not a fitted description of every plant sensor. Real decoders may have several calcium-binding sites, autoinhibition, target-dependent affinity and persistent phosphorylation. Crucially, simple integration of closely spaced pulses does not by itself prove a dedicated frequency code independent of pulse amplitude and duration.
There is experimental evidence that waveform matters. Imposed guard-cell calcium patterns can produce different stomatal outcomes, including a distinction between immediate changes and a maintained response. This goes beyond merely observing that a closing stoma has calcium oscillations. Nevertheless, it establishes a response relationship in a particular experimental system; assigning that relationship to one endogenous decoder requires additional molecular evidence.[ref]
A defined range of guard cell calcium oscillation parameters encodes stomatal movements by G. J. Allen and others. pp. 1053–1057, imposed oscillation parameters and stomatal responses
Likewise, an activated CCaMK can trigger spontaneous nodulation, bypassing upstream requirements. Such bypass experiments place kinase activity downstream of early symbiotic signaling, but do not identify which feature of the native calcium trace the wild-type kinase reads.[ref]Deregulation of a Ca2+/calmodulin-dependent kinase leads to spontaneous nodule development by Leïla Tirichine and others. pp. 1153–1156, spontaneous nodule development after kinase deregulation
Measurement presents a separate limitation. A calcium reporter has its own affinity, response time and dynamic range. Slow reporters can merge brief pulses; saturation can erase amplitude differences. Probe expression can buffer calcium, and population measurements average heterogeneous cells. A calcium signal close to a channel may activate a nearby sensor without creating a large whole-cell change. Comparing different reporters or compartments without calibration can therefore create apparent biological differences that partly reflect measurement.
Finally, decoding depends on state. Sensor abundance, targets, prior phosphorylation, hormones and parallel redox signalling all modify the response to a given calcium signature. Sensors can also regulate channels and calcium removal, feeding back on signal production. A mutant that changes both waveform and output has not cleanly separated encoding from decoding. A decisive study would manipulate relevant waveform features while controlling the others, measure sensor activation and physiological response in the same cells, and test whether selective loss and restoration of decoder function abolish and restore discrimination. The central gap is thus a quantitative causal map linking local calcium dynamics, decoder kinetics and cellular state, rather than a lack of candidate calcium-binding proteins.
Phosphorylation converts ABA perception into regulated ion transport, coordinates calcium-dependent and calcium-independent inputs, and makes stomatal closure reversible. Its role is distributed across a network of kinases, phosphatases and transport targets. ABA does not close the pore by directly supplying a mechanical force.
The opening and closing machinery is a pair of guard cells surrounding a stoma. Accumulation of osmotically active solutes favors water entry and increased turgor pressure; solute loss favors water exit and reduced aperture. During water stress, abscisic acid shifts the balance toward anion and potassium loss. Changes in transport can precede slower changes in gene expression, allowing the existing guard-cell machinery to respond rapidly.
The core ABA switch involves inhibition of an inhibitor. Without the activating ABA signal, selected clade-A protein phosphatase 2C enzymes, including ABI1, restrain ABA-responsive SnRK2 kinases. ABA binding to a PYR-PYL-RCAR ABA receptor promotes inhibition of these phosphatases. This permits activating kinase phosphorylation to persist and supports activation of OST1, also called SnRK2.6. Thus a hormone-dependent change in phosphatase activity changes the phosphorylation state and catalytic activity of downstream signaling proteins. The effect is specific to the relevant receptor, phosphatase and kinase combinations; it is not a claim that all phosphatases inhibit closure or all phosphorylation promotes it.
Biochemical reconstitution supports this causal ordering: defined receptor, phosphatase and kinase components can reconstruct ABA-dependent regulation without requiring an intact plant. This separates a sufficient core perception-and-relay module from the many parallel processes present in a stressed cell. However, a reconstructed molecular or transcriptional readout alone does not prove that the full mechanical response of a stoma has been rebuilt.[ref]
In vitro reconstitution of an abscisic acid signalling pathway by Hiroaki Fujii and others. pp. 660–664, reconstituted ABA signaling components
A crucial transport target is SLAC1. OST1-dependent phosphorylation activates this slow anion channel, allowing anions to leave the guard cell. Anion efflux depolarizes the membrane potential, favoring outward potassium current through GORK. Loss of these solutes reduces the osmotic drive retaining water, so water exits and turgor pressure falls. Activation of an anion channel can therefore initiate a larger electrical and osmotic response without the kinase phosphorylating every ion that moves. Suppression of opening-associated transport further reinforces the shift toward closure.
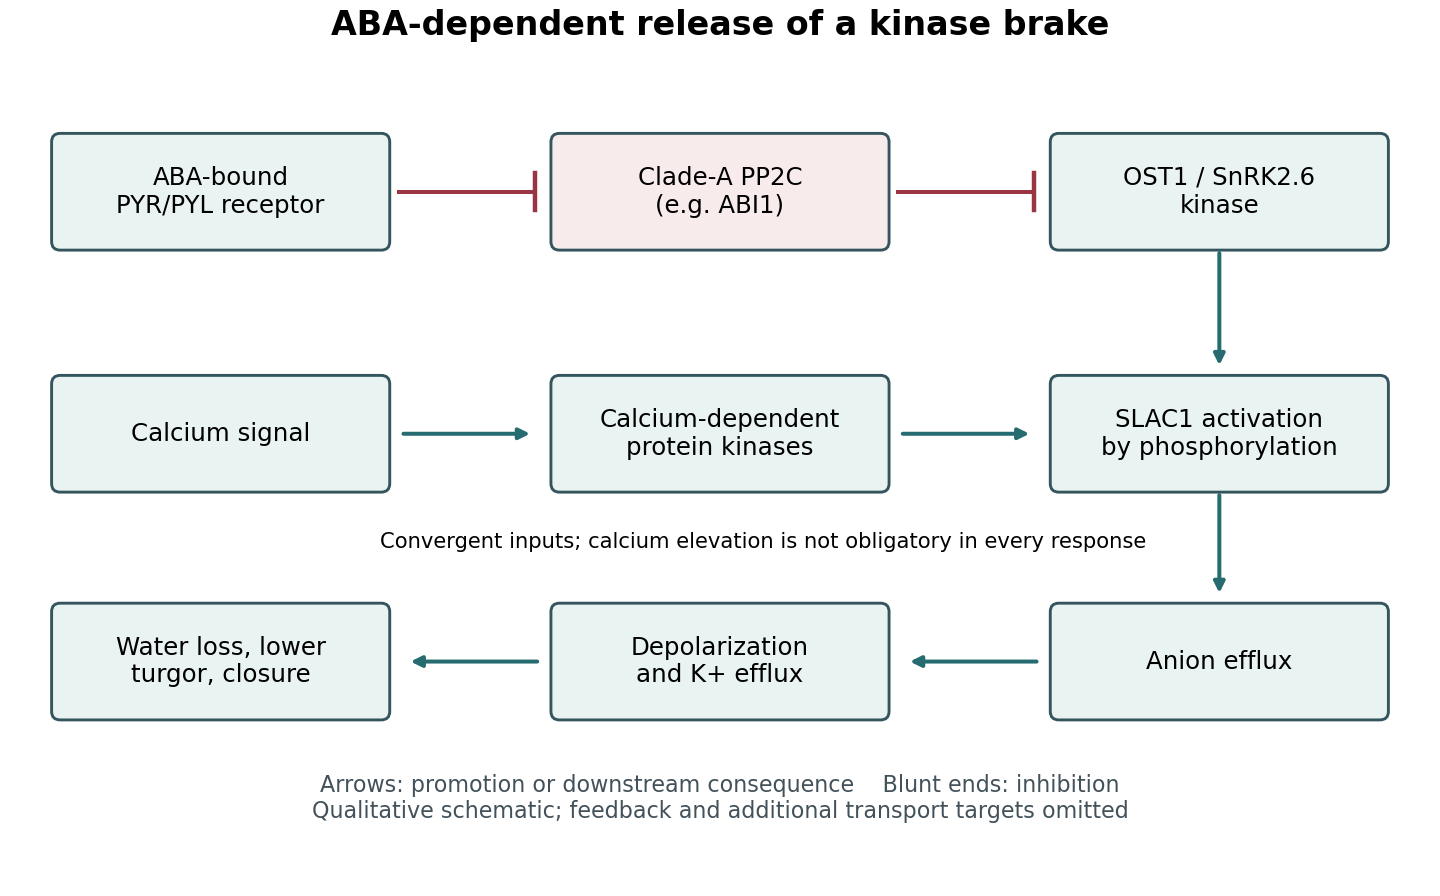

Channel activation experiments provide an important bridge between the core ABA switch and physiology. Coexpression and electrophysiology showed that OST1 activates SLAC1, whereas phosphatase action antagonizes activation; kinase activity and channel regulatory regions are therefore functionally important. These findings are stronger than simple colocalization. Together with guard-cell genetic and current measurements, they support a route from a phosphorylation-dependent channel change to altered aperture. A heterologous cell nevertheless lacks the complete transport and mechanical environment of a real guard cell.[ref]
Activity of guard cell anion channel SLAC1 is controlled by drought-stress signaling kinase-phosphatase pair by Dietmar Geiger and others. Figures 1–4, channel currents and kinase–phosphatase regulation
Calcium-dependent signaling converges on this machinery. Calcium-dependent protein kinases can activate SLAC1, and different kinases have different calcium sensitivities. Consequently, phosphorylation can combine hormone-dependent release of the phosphatase brake with a calcium signature. This is a convergence network, not a mandatory linear sequence in which ABA must always cause a measurable global calcium rise before any closure can occur.[ref]
Guard cell anion channel SLAC1 is regulated by CDPK protein kinases with distinct Ca2+ affinities by Dietmar Geiger and others. pp. 8023–8028, kinase-specific calcium dependence and anion-channel regulation
Regulation of plant NADPH oxidases and reactive oxygen species can further couple kinase activity, redox signalling and calcium entry. The physiological contribution of these branches varies with conditions.Reversal is as important as activation. Phosphatases, calcium clearance and renewed opening-associated transport reset the system when conditions change. Phosphorylation can alter activity, interactions and localization without waiting for protein replacement. The outcome is a tunable balance of kinase and phosphatase activities that connects ABA-dependent sensing to solute flux, water movement and pore mechanics, while integrating additional environmental inputs.
Plants use an entrained circadian clock to change their sensitivity to stimuli, while also responding directly to the current light and temperature environment. The same external stimulus can therefore have different effects at different internal phases. This circadian gating must be distinguished from a daily rhythm caused solely by daily variation in the stimulus itself.
The plant circadian clock contains interlocking regulation of gene expression, protein accumulation and protein activity. Morning-associated regulators such as CCA1 and LHY interact with later-acting components, including TOC1, to generate a sequence of phases rather than a single daily on–off switch. Light information, including inputs involving phytochromes and cryptochromes, and temperature cues adjust the clock through entrainment of circadian rhythm. Under suitably constant conditions, a free-running circadian rhythm persists. Anticipation of dawn or dusk is therefore possible before the corresponding environmental transition occurs.
Clock outputs can modify several points in a stimulus-response pathway. A receptor or transport protein may accumulate at a particular phase; signaling inhibitors may be removed at another. The clock can regulate hormone production, hormone inactivation, transport and sensitivity of downstream transcription factors. Post-translational regulation allows a phase-specific transcript to produce an output only under a second permissive condition. Consequently, a rhythmic hormone concentration and rhythmic responsiveness to that hormone are distinct explanations and may coexist.
Auxin provides direct experimental evidence for sensitivity gating. Timed auxin treatments and transcriptional reporters in Arabidopsis showed that an externally supplied hormone stimulus produces phase-dependent responses; growth responses were also gated. Because the stimulus was supplied experimentally, the result cannot be explained merely by assuming that the plant normally makes more auxin at one time of day. Reporter dynamics and pretreatment baselines still require appropriate controls, and a reporter is not a direct measurement of free hormone.[ref]
An illustrative local description iswhere is a small standardized stimulus, is circadian phase and is the response above the matched untreated baseline. A phase-dependent gain represents gating. In contrast, if is constant but the baseline response oscillates, observing different absolute values after treatment does not establish gating. Real pathways can saturate or change sign, so this equation illustrates the experimental distinction rather than defining a universal linear law.
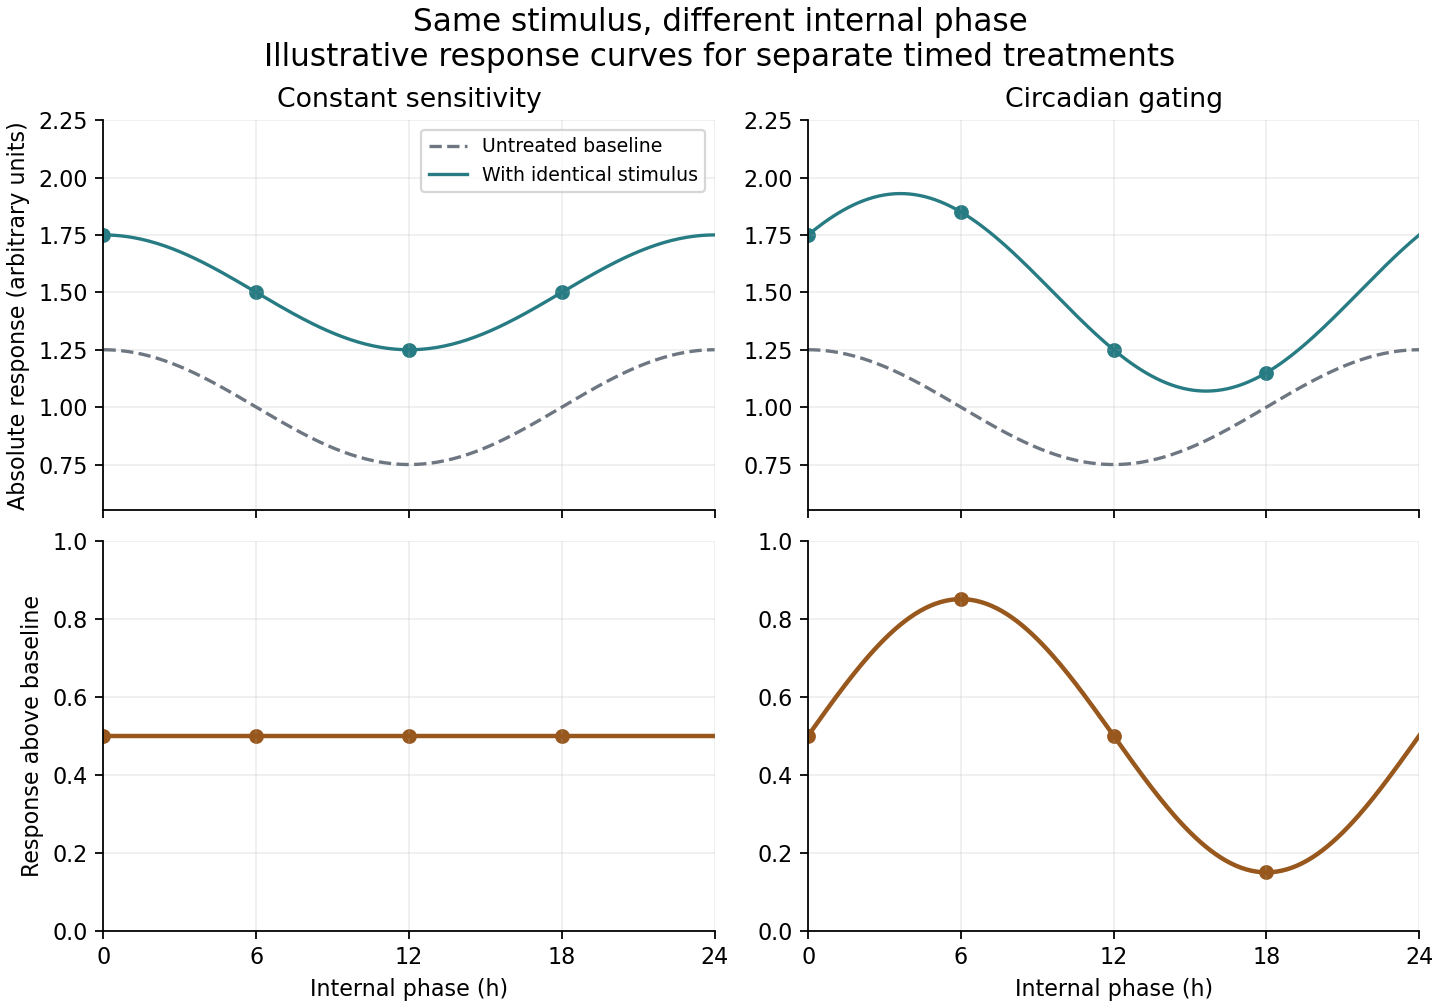
Phase-dependent sensitivity differs from a rhythmic untreated baseline
. Original stipulated model, not experimental data. Identical stimulus pulses give equal baseline-subtracted responses in the constant-sensitivity example, but unequal responses when sensitivity is gated by circadian phase. The selected amplitudes and phase have no fitted biological meaning. Details.
Photoperiodism shows how internal time can be combined with an external cue to produce a developmental decision. In Arabidopsis, timed expression of CONSTANS interacts with light-dependent regulation of the protein. In long days, a permissive expression phase overlaps light sufficiently to support FLOWERING LOCUS T activation. The external coincidence model therefore responds to when light occurs relative to the clock, rather than merely adding up photons. Photoreceptor-dependent protein regulation provides a molecular connection between timing and the external environment.[ref]
Photoreceptor regulation of CONSTANS protein in photoperiodic flowering by Federico Valverde and others. pp. 1003–1006, light regulation of CONSTANS and photoperiodic flowering
FT protein can then communicate from leaves to the shoot apex. Phloem-specific expression and grafting experiments support FT protein movement as part of this long-distance floral signal.[ref]FT protein movement contributes to long-distance signaling in floral induction of Arabidopsis by Laurent Corbesier and others. pp. 1030–1033, mobile FT protein and floral induction
A convincing demonstration of circadian gating compares matched stimuli at several internal phases under constant external conditions, with untreated controls at every phase. Plants entrained to opposite schedules can help distinguish internal phase from laboratory clock time. Clock perturbations and restoration of clock function strengthen causal interpretation, provided effects on general health and growth are considered. A phase-shifted response in constant conditions supports clock control; disappearance immediately when the environmental cycle is removed suggests direct environmental control, although weak rhythms and altered physiology can complicate that inference. Masking of circadian rhythm, in which an environmental cue directly changes a measured output, can coexist with clock control.
Timing is useful because demands and risks recur. Coordinating stomatal conductance, photosynthetic preparation and growth with expected light availability can improve resource use. Yet the optimum phase depends on temperature, water availability and day length, and a strong acute stress can override a normal daily preference. Plants combine an internal estimate of time with current conditions, changing pathway sensitivity as well as the abundance of signals and response machinery.
Plant developmental plasticity is achieved by making growth-regulatory machinery depend jointly on environmental inputs, hormone state, spatial information and internal time. Integration can occur through direct protein interactions, regulated protein turnover, transport of a second signal or convergence on gene expression. Evidence is strongest when it identifies the shared molecular step and connects that step to an altered developmental response.
A useful starting distinction is between plasticity and genetic adaptation. A genotype can produce different root or shoot architectures in different environments without acquiring a new mutation. Such phenotypic plasticity may be beneficial, neutral or costly. Moreover, an induced developmental decision need not be reversible after a tissue or organ forms. Integration therefore regulates the trajectory and allocation of future growth, rather than simply toggling every mature structure between two interchangeable states.
Light and gibberellin provide a well-resolved example. Growth-promoting phytochrome-interacting factors regulate elongation-associated genes. Active phytochrome signaling can reduce the abundance or activity of these factors, restraining elongation under appropriate light conditions. Meanwhile, low gibberellin signaling permits accumulation of DELLA proteins; gibberellin perception promotes their destruction through regulated protein degradation. The two inputs meet because DELLA proteins can bind growth-regulatory PIFs, including PIF4, and restrict their DNA-binding activity. Light-regulated PIF availability and hormone-regulated DELLA restraint jointly determine access to growth targets.
The evidence is not simply that light and gibberellin affect the same seedling phenotype. Protein-interaction and DNA-binding analyses, interpreted alongside genetic growth phenotypes, link DELLA–PIF4 association to inhibition of transcription-factor function. Removing a growth restraint can therefore increase elongation only insofar as the necessary growth-promoting machinery and resources remain available. This explains why the output of one pathway depends on the state of the other.[ref]
A molecular framework for light and gibberellin control of cell elongation by Miguel de Lucas and others. pp. 480–484, DELLA interaction with PIF4 and effects on DNA binding and elongation
It would be an overstatement to treat every PIF or every light response as identical: family members differ, and transcription-factor availability is only one constraint on growth.This architecture can behave like a permissive gate. If effective PIF activity is low, removal of DELLA repression alone may produce little output; if DELLA inhibition is strong, abundant PIF may still fail to activate its targets. The biological gate is graded rather than an exact Boolean operation, because protein concentrations, binding affinities and competing interactions vary. The important point is that the joint response need not equal the sum of two independent responses. A shared physical interaction supplies a mechanism for that non-independence.
Roots illustrate integration through transport rather than only transcription-factor binding. NRT1.1 connects the nutrient nitrate to auxin distribution. At low nitrate, its auxin-transport activity can favor removal of auxin from developing lateral roots, restricting their growth. Nitrate inhibits this transport activity, allowing a different local auxin distribution and a different developmental outcome. Mutant phenotypes and transport measurements connect a nutrient-responsive membrane protein to hormone transport and root architecture.[ref]
Nitrate-regulated auxin transport by NRT1.1 defines a mechanism for nutrient sensing in plants by Gabriel Krouk and others. pp. 927–937, nitrate-dependent auxin transport and lateral-root responses
The mechanistic claim is specific: local nitrate can regulate a route affecting local auxin accumulation. It does not establish that raising nitrate indefinitely always increases branching, or that whole-plant nitrogen status is irrelevant.Spatial organization matters because a root encounters patches rather than one uniform nutrient concentration. Polar auxin transport can turn a local input into a developmental distribution of hormone, while whole-plant nutritional and carbon status constrain how much growth is affordable. A transporter can thus perform both acquisition and regulatory functions. Conversely, a transport-deficient mutant may change nutrient supply as well as signaling. Separating these effects requires measurements of transport, hormone distribution and development, rather than interpreting altered growth alone as proof of a dedicated sensor function.
Time adds another dimension. Circadian gating of auxin responses means that equal hormone input can have different transcriptional and growth consequences at different internal phases. This can coordinate an environmentally favorable growth opportunity with a phase when the growth machinery is permissive.[ref]
The Circadian Clock Regulates Auxin Signaling and Responses in Arabidopsis by Michael F. Covington and others. Figures 4–5, phase-dependent responses to supplied auxin
Again, joint regulation is more informative than merely finding two pathways with overlapping lists of expressed genes.Causal tests should ask whether disrupting the proposed connection specifically changes the interaction between inputs. A binding-defective regulator, a transport perturbation or a suitable rescue can distinguish direct integration from parallel downstream consequences. Epistasis helps order requirements, but a severe growth defect can conceal an otherwise independent response. The convincing picture is therefore a network of identifiable biochemical junctions, illustrated by DELLA–PIF interactions and nitrate-dependent auxin transport, whose spatial and temporal deployment converts environmental information into plastic development.
Plants cope with changing light by combining rapid feedback from the photosynthetic apparatus, photoreceptor-controlled movements and slower acclimation. The problem is to preserve reaction centers during excess excitation while recovering productive light use when the excess disappears. Changes in intensity and changes in spectral balance require overlapping but distinct responses.
A sunfleck can increase excitation faster than carbon assimilation adjusts. If electron acceptors or metabolic use become limiting, continued excitation increases the risk of damaging reactions and reactive oxygen species. Rapid photoprotection therefore regulates both excitation delivery and electron flow. This is not equivalent to maximizing fluorescence quenching at every moment: energy safely dissipated during high light becomes an opportunity cost if dissipation persists after a return to shade.
An important feedback signal is acidification of the thylakoid lumen as photosynthetic electron transport builds a proton gradient. Proton-dependent changes involving PsbS and antenna organization promote rapidly reversible components of non-photochemical quenching. The xanthophyll cycle also contributes: conditions favoring de-epoxidation toward zeaxanthin support protective energy dissipation. Excess absorbed excitation can then be released as heat rather than entering potentially damaging photochemistry. As light falls and the proton gradient relaxes, dissipation should decrease, although different components recover on different timescales. Loss-of-function analysis of PsbS separated its quenching role from basic light capture.[ref]
A pigment-binding protein essential for regulation of photosynthetic light harvesting by Xiao-Ping Li and others. pp. 391–395, PsbS requirement for regulated quenching
The physiological importance of recovery kinetics is experimentally testable. Accelerating recovery from photoprotection in tobacco increased carbon uptake and dry-matter production under fluctuating light. The experiment supports the proposition that delayed relaxation can constrain productivity; it does not imply that eliminating protection would be beneficial or that an identical yield improvement is guaranteed in every crop and environment.[ref]
Improving photosynthesis and crop productivity by accelerating recovery from photoprotection by Johannes Kromdijk and others. pp. 857–861, modified photoprotective recovery and tobacco productivity
Protection and productive capture must be optimized jointly.Spectral imbalance creates a second problem: photosystem I and photosystem II may receive unequal excitation. The redox state of the intersystem electron-transfer machinery can regulate STN7 kinase, which phosphorylates a mobile fraction of LHCII. Photosynthetic state transitions thereby redistribute antenna excitation between the photosystems. This reallocates excitation rather than simply dissipating it as heat. Genetic loss of STN7 disrupts state transitions, connecting a specific kinase to the adjustment.[ref]
State transitions and light adaptation require chloroplast thylakoid protein kinase STN7 by Stéphane Bellafiore and others. Figure 1 and pp. 892–895, STN7-dependent state transitions
Their contribution depends on the spectral and physiological setting; state transitions should not be presented as the sole explanation of all responses to fluctuating sunlight.Regulation also acts on electron delivery. Cyclic electron flow around photosystem I can support proton-gradient formation without net NADPH production, helping adjust ATP supply and protective regulation. Lumen-dependent photosynthetic control can restrict delivery through the cytochrome b6f complex, protecting downstream acceptors against excessive reduction. The PGR5-associated route is important in this regulation; mutant evidence links it to photoprotection, while not requiring the claim that PGR5 alone is a complete electron-transfer enzyme.[ref]
A plant also senses light before damage occurs. Phototropins are blue-light receptor kinases controlling responses including chloroplast relocation and stomatal opening. Under weak light, positioning chloroplasts to intercept more light can aid capture; strong-light avoidance reduces direct exposure. Avoidance-defective Arabidopsis mutants identified a phototropin-related receptor as a requirement, providing evidence for a signaling mechanism rather than passive displacement by light.[ref]
Arabidopsis NPL1: a phototropin homolog controlling the chloroplast high-light avoidance response by Takatoshi Kagawa and others. pp. 2138–2141, avoidance mutants and receptor identification
Coordinating stomatal conductance with light also changes carbon dioxide supply, but carries a water-loss cost and interacts with ABA-dependent closure.Over longer periods, phytochrome and cryptochrome signaling can alter growth and leaf development, while chloroplast-derived retrograde signaling helps coordinate nuclear responses with organelle state. Photosynthetic acclimation changes antenna investment, electron-transfer capacity and metabolic capacity. These slower changes complement rapid regulation of existing proteins. Damage still occurs: photosystem II repair, including replacement of damaged D1 protein, restores capacity when prevention is incomplete. Persistent photoinhibition should be distinguished from reversible protective quenching.
The integrated solution uses several timescales: rapid lumen and redox feedback for safe operation, photoreceptors for light-dependent positioning and gas exchange, and acclimation and repair for sustained performance. Demonstrating success requires carbon gain, growth and damage measurements under realistic fluctuations; one fluorescence parameter alone cannot identify every pathway or establish improved productivity.
Engagement with beneficial microorganisms is a regulated allocation decision: plants combine partner signals with nutrient demand, immune control and whole-plant feedback, then adjust investment according to the association's performance. Recognition, entry, organ development and continued nutrient exchange are separate control points. A compatible signal is evidence of partner identity or capability, not a guarantee of future benefit.
Legume–rhizobial symbiosis illustrates early selectivity. Root-exuded flavonoids can induce production of rhizobial Nod factors. Compatible plant receptors recognize these lipochitooligosaccharides and initiate signaling that permits infection and root nodule development. Structural specificity of the signals and the host receptor repertoire constrain compatibility. Meanwhile, plant immunity must be coordinated with accommodation: unrestricted entry would be costly, but an indiscriminate defense response would prevent the mutualism. This is a conditional developmental program, not a complete abolition of defense.
Early symbiotic signaling includes nuclear calcium signatures and activation of CCaMK within the common symbiosis signaling pathway. Kinase activation connects early perception to downstream transcription and developmental responses. Deregulated CCaMK can induce spontaneous nodules, demonstrating that downstream developmental machinery can be activated without the normal upstream sequence. A spontaneous nodule is nevertheless not evidence of bacterial entry or effective nitrogen fixation; the latter requires additional coordinated functions.[ref]
Deregulation of a Ca2+/calmodulin-dependent kinase leads to spontaneous nodule development by Leïla Tirichine and others. pp. 1153–1156, bypass of upstream requirements and spontaneous organ development
Arbuscular mycorrhiza uses a partly shared signaling apparatus but a different exchange structure and different partners. Plant strigolactones released into the rhizosphere stimulate fungal branching, increasing the potential for contact. Isolation of a root-exuded branching factor and chemical identification as a strigolactone connected a specific plant molecule with fungal behavior.[ref]
Plant sesquiterpenes induce hyphal branching in arbuscular mycorrhizal fungi by Kohki Akiyama and others. pp. 824–827, identification of the branching factor and fungal responses
Subsequent recognition and intracellular accommodation depend on host signaling and cell remodeling. Sharing a calcium-linked pathway does not mean that fungi are recognized by the same Nod-factor receptors as rhizobia, or that every beneficial root bacterium uses this pathway.Nutritional context changes the expected return. A plant with adequate available nitrogen has less reason to spend photosynthate on additional nitrogen-fixing nodules. Similarly, high phosphate availability commonly reduces investment in arbuscular mycorrhiza. Hormone and nutrient pathways can alter signal release, developmental competence and allocation. Carbon availability matters as well: the plant must supply carbon to sustain the association. These controls act on potential benefit and cost rather than classifying one microorganism as beneficial under all conditions. A symbiont can be compatible yet provide little net growth advantage in a particular environment.
Local permissiveness must also be coordinated across a branched root system. Autoregulation of nodulation provides systemic negative feedback. Signals from an initiating symbiosis include root-produced CLE peptides; shoot receptor-kinase pathways involving HAR1 in Lotus japonicus contribute to limiting further engagement. A shoot-to-root arm involves miR2111, which represses the root negative regulator TML. Reduced delivery of this permissive microRNA allows the brake to rise. Thus stopping further infection can be achieved by withdrawing repression of a repressor, rather than by sending a simple mobile toxin to all root tips. Experiments established shoot-to-root movement of miR2111 and its role in controlling infection through TML.[ref]
Systemic control of legume susceptibility to rhizobial infection by a mobile microRNA by Daniela Tsikou and others. pp. 233–236, mobile miR2111, TML and systemic symbiotic susceptibility
Particular receptor and peptide names vary among legumes; the Lotus mechanism should not be transferred gene-for-gene to every plant.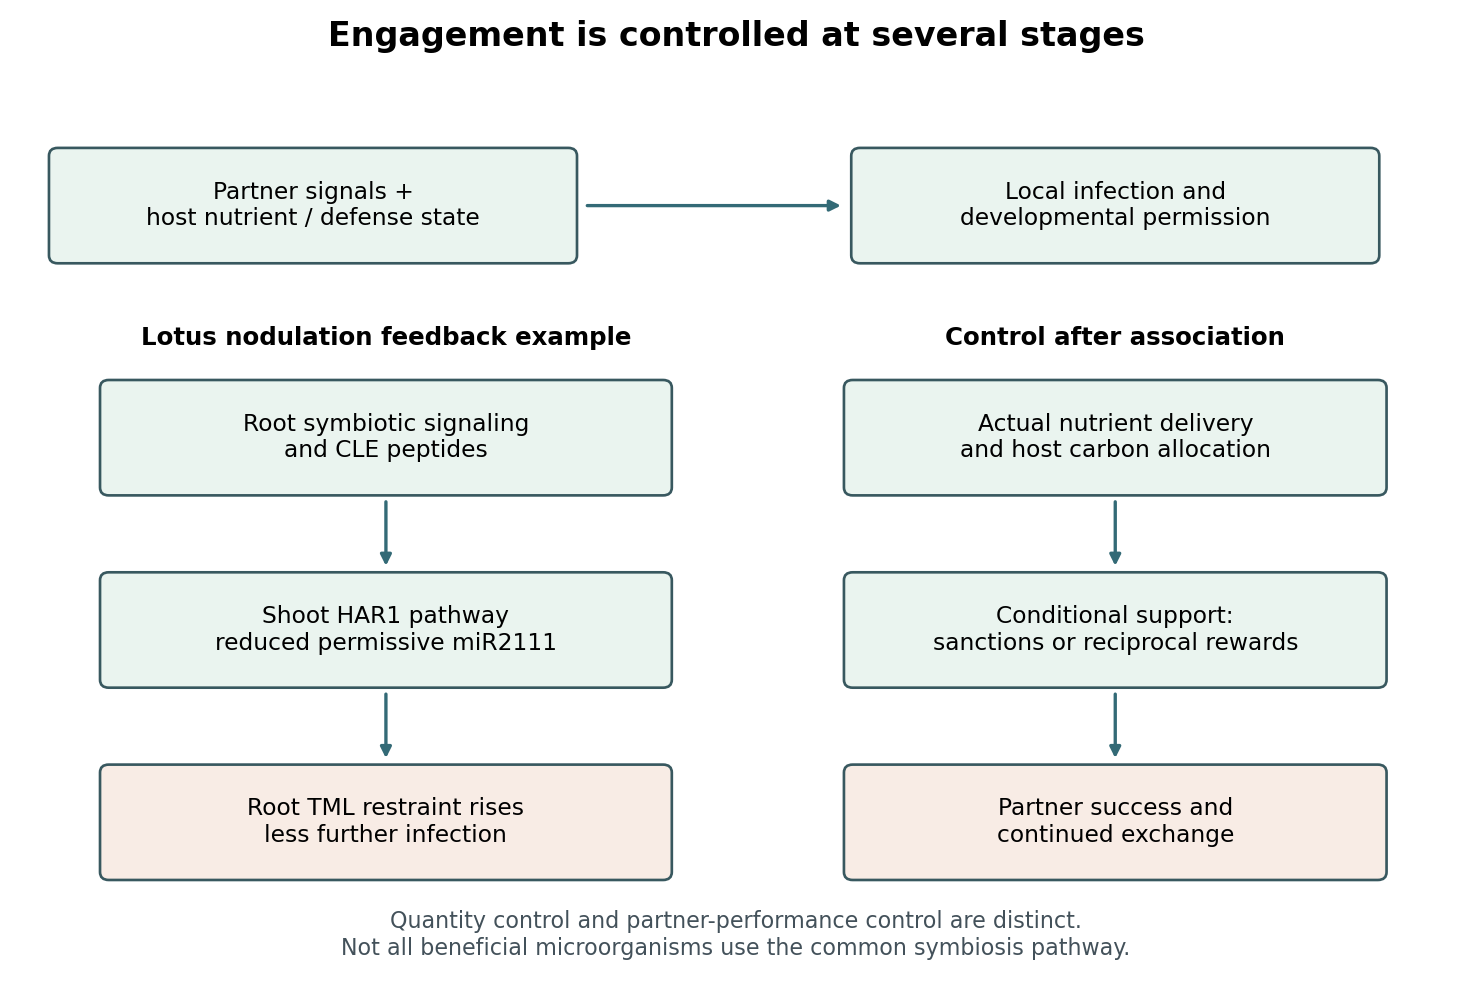
Local partner recognition, systemic quantity control and conditional resource allocation
. Original conceptual diagram. The Lotus nodulation feedback example is distinguished from later partner-performance control. AON limits further engagement, whereas sanctions and reciprocal rewards act on resource allocation or symbiont success after association. The diagram does not imply that all beneficial microorganisms use the nodulation pathway. Details.
Systemic quantity control is distinct from assessment of an established partner's performance. In soybean, experimentally preventing an otherwise mutualistic rhizobium from fixing nitrogen reduced its reproductive success. Nodule oxygen measurements implicated reduced oxygen supply as a possible sanction mechanism. Because cooperation was changed by removing molecular nitrogen from the atmosphere, the comparison helped separate fixation performance from unrelated differences between bacterial strains. It still does not show that every inefficient symbiont is perfectly detected or that oxygen supply is the only possible control.[ref]
Host sanctions and the legume-rhizobium mutualism by E. Toby Kiers and others. pp. 78–81, especially Figures 2–3, suppressed fixation, reproductive success and oxygen relations
In mycorrhizal exchange, resource allocation can be conditional on both sides. Experiments demonstrated increased plant carbon allocation toward more cooperative fungal partners and increased fungal nutrient allocation in response to carbon supplied. This supports reciprocal reward in symbiosis, rather than a model of unlimited plant command over a passive fungus.[ref]
Reciprocal rewards stabilize cooperation in the mycorrhizal symbiosis by E. Toby Kiers and others. pp. 880–882, experimental manipulation of partner cooperation and allocation
Host sanctions, partner choice before entry and reciprocal rewards are therefore related but distinguishable routes to maintaining benefit.Plants regulate engagement through successive filters: compatibility and defense at entry, developmental and nutritional permission, systemic feedback on quantity, and conditional support of established partners. Experiments should score infection, nodule or arbuscule abundance, actual nutrient transfer and host growth separately. A greater colonized area or larger nodule count alone does not prove a more beneficial association.
Articles by others on the same topic
There are currently no matching articles.